

Submitted:
31 October 2026
Posted:
03 November 2026
You are already at the latest version
Abstract
The future of developmental population neuroscience lies in transforming the path to brain individuality into personalized, context‑sensitive, and actionable predictions.
Keywords:
brain chart
; lifespan
; brainality
; epigenetics
; brainnet
; epibrainnetics
Sixteen years ago, Tomas Paus formally articulated Population Neuroscience as an integrative framework that bridges neuroscience, genetics, and epidemiology to uncover factors shaping the human brain (1). Over the past decade and a half, the explosive growth of large-scale neuroimaging datasets combined with advances in analytical methods, has propelled the field far beyond its initial scope. A particularly fertile direction has emerged along the developmental dimension of the human lifespan, giving rise to what we now call Developmental Population Neuroscience (2). This subfield leverages population-based sampling, longitudinal designs, and multilevel data (from genes and molecules to circuits, behaviour, and community contexts) to map the development of normative brain trajectories and identify sources of individual variation across development (3). Yet, despite remarkable empirical progress (4), the field still lacks a unifying biophysical framework that can coherently link processes operating at vastly different scales, from molecular gradients and synaptic pruning to social environments and cultural embedding. Such a framework is urgently needed to move Developmental Population Neuroscience from descriptive curve-fitting towards a mature, predictive discipline capable of generating mechanistic insights and guiding targeted interventions.
In 1942, the developmental biologist Conrad Hal Waddington introduced a metaphor that has shaped developmental biology for generations (5). He imagined a ball rolling down a landscape of hills and valleys. At the summit stands a pluripotent cell, brimming with potential. As the ball descends, it encounters branching valleys. Each fork is a developmental turning point. The valley walls, steep and protective, channel the ball toward a specific fate, ensuring that despite genetic noise and environmental perturbations, the embryo reliably becomes a healthy organism. Waddington called this buffering capacity canalization, and his model of the epigenetic landscape illustrated how development achieves robustness without deterministic pre-specification. It describes a process that takes place largely before birth. The ball’s trajectory is determined by the shape of the landscape, which is prespecified by the genetic makeup of the organism, though the chosen path can be altered by extrinsic events. The organism does not choose its path; the path chooses the organism. And when the ball finally comes to rest in a deep valley, development is complete. The journey ends.
Human brain development tells a different story. Unlike cell differentiation, which largely finishes before birth, the human brain undergoes an extraordinarily protracted period of postnatal maturation, lasting well into the third decade of life and beyond (6). Cortical gray matter volume peaks around age 6 and then declines, while white matter volume increases steadily through adolescence and into young adulthood. Synaptic density in the prefrontal cortex does not reach its peak until after the first year of life and does not reach adult levels until the third decade. Myelination of association cortices continues into the second decade, and cortical thinning accelerates during adolescence before gradually stabilizing. These are not the dynamics of a ball rolling passively toward a predetermined basin. They are the dynamics of a system that is actively sculpted by experience, choice, and interaction.
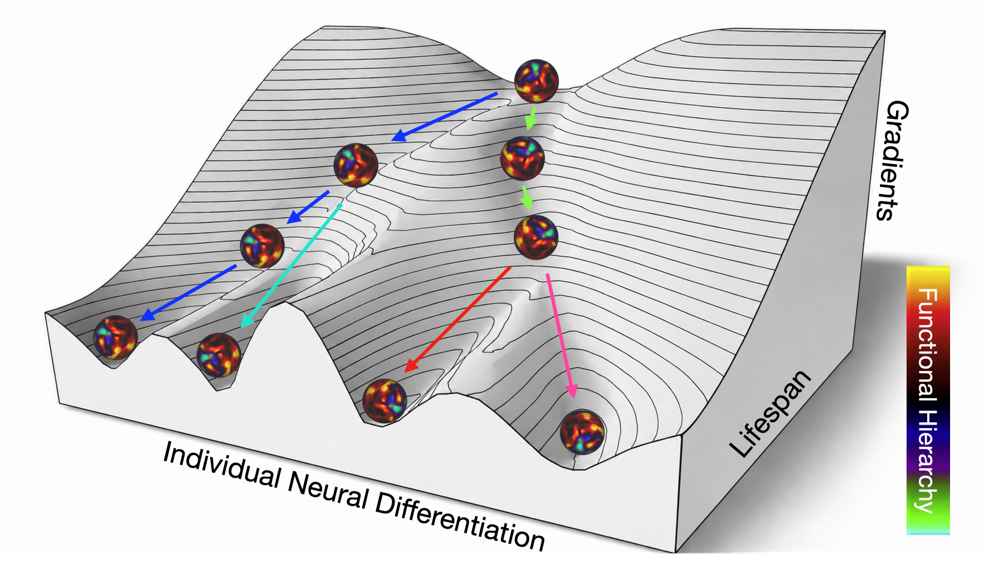
Here, we revise the Waddington landscape by replacing the cell with the brain and delineating its structure from three dimensions: gradients, lifespan, and individual neural differentiation (Figure 1a). This landscape of the path to brain individuality or brainality landscape is introduced for Developmental Population Neuroscience to achieve biophysical modeling of human neurodevelopment at different scales across the life span.
Gradients as the Driving Force of Landscape Organization
Central to the brainality landscape is the concept of functional connectivity (FC) of the whole human brain network (brainnet) or connectome. It refers to the temporal correlation of spontaneous low-frequency fluctuations measured across spatially distinct brain regions (7,8). These intrinsic correlations reveal the brain’s large-scale functional architecture without requiring any explicit task, and they are present even in the absence of conscious awareness, as demonstrated in anaesthetized animals (9). Over the past three decades, FC has enabled the reliable identification of multiple reproducible large-scale brainnets such as default and salience ventral attention networks that recapitulate spatial topographies observed during task-evoked activity (10-13). Importantly, individual differences in FC are stable over time and can serve as “fingerprints” for identifying individuals (14-15). These properties make FC a powerful lens for mapping the normative and atypical trajectories of brain development and provide the empirical foundation for the gradients and brain charts that follow in the landscape.
The foundational insight that cortical organization can be understood through large-scale spatial gradients emerged from the observation that functional connectivity does not fall into discrete, sharply bounded parcels but rather varies continuously across the cortical sheet. A landmark study (16) identified a principal gradient spanning from primary sensorimotor areas at one end to regions of the default network at the other. This gradient captured the dominant axis of variance in functional connectivity patterns and was shown to be phylogenetically conserved in the macaque monkey, suggesting that it reflects a fundamental organizing principle of primate cortical architecture. Converging evidence from microstructure, connectivity, and gene expression formalized the sensorimotor-to-association (SA) gradient as a core organizational axis of the human cerebral cortex (17).
Recent advances have deepened our understanding of this axis across multiple scales. At the molecular and cellular scale, integrated whole-brain spatial transcriptomics, magnetic resonance imaging (MRI), and retrograde tracing in the marmoset monkey discovered an opposing molecular gradient axis that underlies primate cortical organization (18). One gradient emanates from allocortical and periallocortical regions (e.g., piriform and entorhinal cortices), whereas the opposing gradient originates from primary sensory areas, with association cortices residing at their intersection. This axis is present at birth but undergoes prominent postnatal refinement, suggesting that it is actively shaped by sensory experience. Such molecular axis is mirrored in thalamic gene expression and aligns with thalamocortical connectivity, indicating that the SA axis is not merely a cortical phenomenon but reflects a coordinated cortico-subcortical organizational rule. Gene ontology reveals that the SA axis is enriched for synaptic signaling and vesicle-cycle genes, with gene-gradient coupling peaking early in life and declining into adulthood, consistent with a transient genetic scaffold for early functional differentiation.
From an evolutionary and developmental perspective, the multimodal induction-exclusion in network development model demonstrates that the SA axis is shaped by competing molecular programs (19): a central program induced by first-order thalamocortical inputs that establishes primary sensorimotor areas, and a pericentral program emerging from the frontotemporal poles that defines higher-order association cortex. These two programs antagonistically interact, with the pericentral program expanding inward while being excluded from primary territories. Key effector molecules such as SEMA7A (enriched in primary areas) and PLXNC1 (enriched in association cortex) mediate mutual axonal repulsion between primary and association cortices, providing a mechanistic basis for the topographic segregation captured by the SA gradient. Notably, this opposing gradient architecture is evolutionarily conserved across birds, marsupials, and primates, suggesting that it represents an ancient organizational motif that has been co-opted and elaborated during cortical expansion.
At the macro-scale level of human neuroimaging, the canonical SA axis exhibits a protracted inverted-U-shaped lifespan trajectory revealed by the first continuous normative atlas of functional connectome gradients from birth to 100 years of age (20): its range expands across infancy, childhood and adolescence, peaking in early adulthood (≈18.8 years), before contracting during ageing. The fidelity of an individual’s SA gradient to the population template is robustly associated with cognitive performance across multiple domains, from fluid intelligence to processing speed and memory, and this association consolidates with age. Moreover, structure–function correlation along the SA axis decreases nonlinearly across the lifespan, with the most rapid decoupling occurring during infancy and early childhood (21-23), suggesting that early functional organization is more tightly tethered to microstructural scaffolds, whereas mature hierarchies become increasingly driven by distributed patterns of functional co-activation.
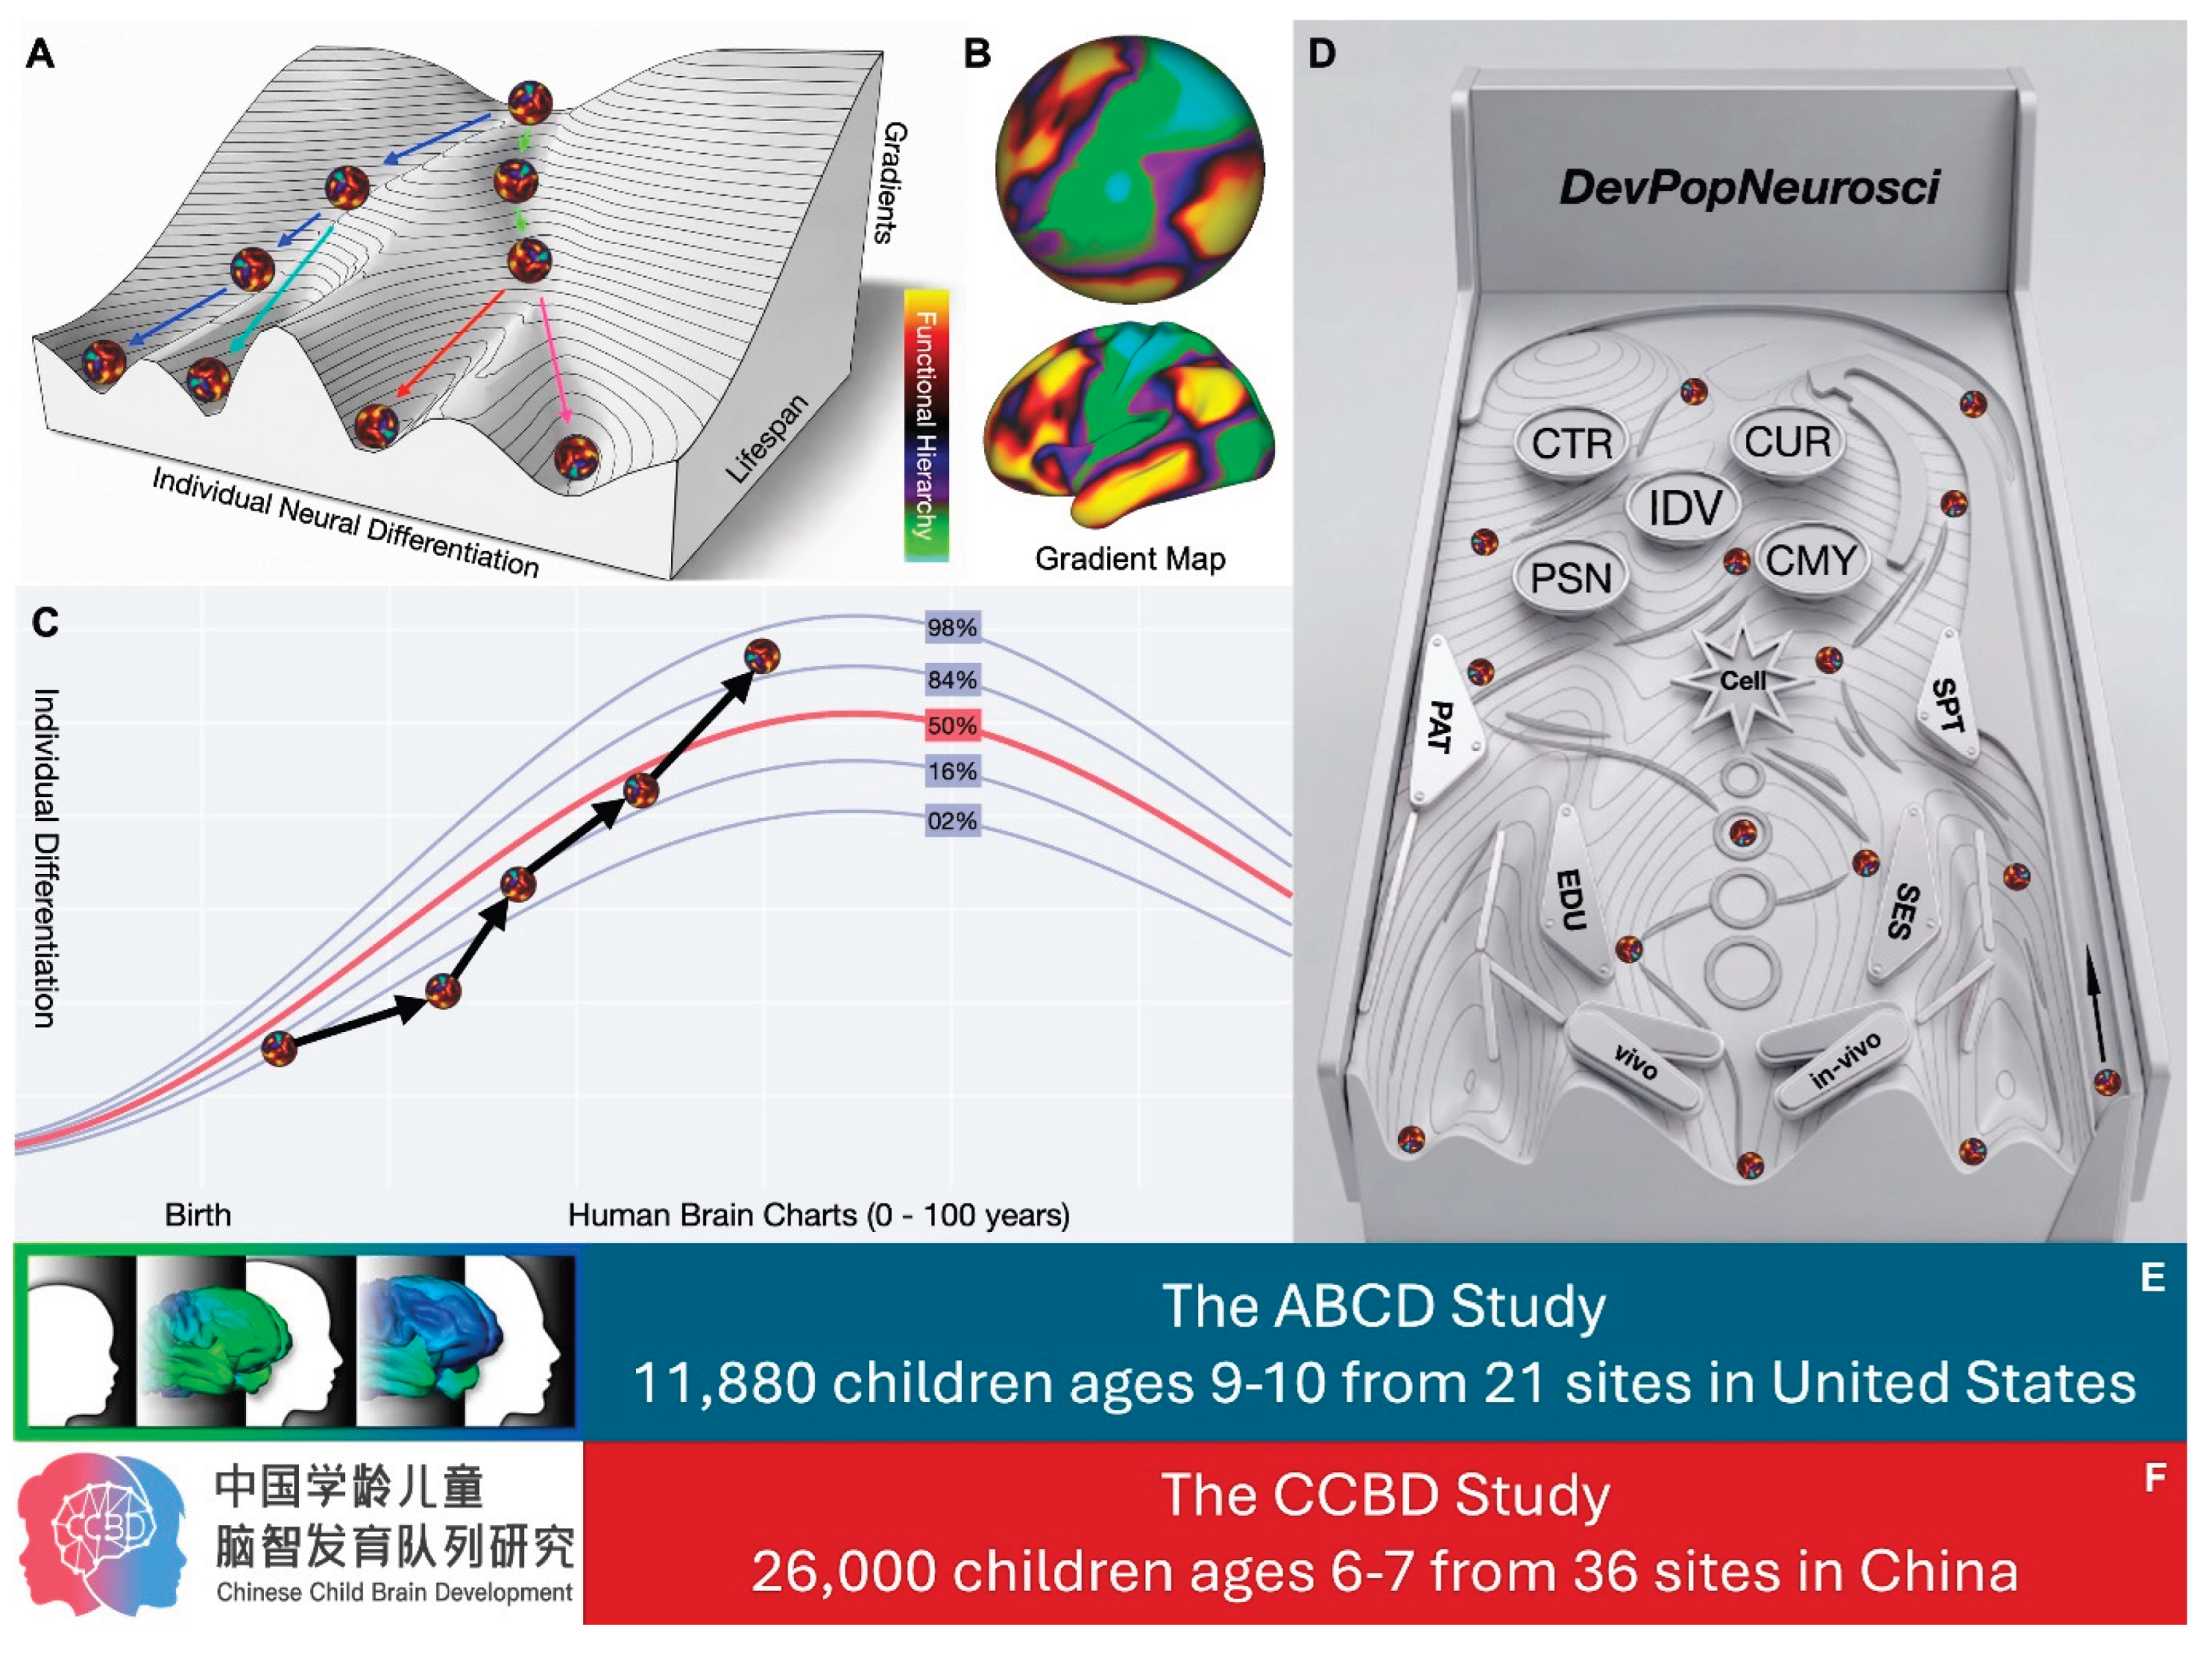
These converging lines of evidence, from molecular transcriptomics, evolutionary developmental biology and lifespan connectomics, establish the SA gradient as the primary axis of human cortical hierarchy. It is not a static topographic feature but a dynamic, multi-scale organizing principle that serves as a driving force propelling the human brain along its developmental trajectory toward the frontier of higher-order cognition (Fig. 1b). The SA axis captures the progressive differentiation from perception and action to abstraction and integration, and its normative trajectory across the lifespan provides a quantitative scaffold for understanding both typical neurodevelopment and its deviations in neuropsychiatric disorders (6). The gradient dimension thus provides a spatial coordinate system that links molecular identity, cellular composition, and functional specialization, offering a biological substrate for the topographic features of Waddington's original landscape, which we refer to as the brainality landscape.
Lifespan Brain Charts and Individual Differentiation
Given the immense complexity of neurodevelopmental diversity at the individual level across the entire human lifespan, a unifying methodological framework is required to reconcile general population laws with personalized trajectories. Brain charts provide precisely such a framework. They extend Waddington’s classic epigenetic landscape metaphor by translating the abstract concept of canalized developmental channels into an empirical, data-driven visualization. In this view, brain charts do not merely summarize group averages; they integrate two orthogonal dimensions of the brainality landscape, lifespan (the temporal unfolding of normative trajectories) and individual neural differentiation (the extent to which each individual deviates from, or converges toward, the population-level channel). By doing so, brain charts transform the static valley-and-ball imagery into a dynamic, quantifiable atlas of human brain development.
The methodological groundwork for brain charts was laid through efforts to establish reliable, scalable pipelines for macroscale connectome discovery (see 24 for a review). Using generalized additive models for location, scale and shape (GAMLSS), Connectome Computation System (25) demonstrated the feasibility of delineating normative trajectories of cortical thickness and surface area across seven large-scale functional networks, highlighting distinct developmental and aging patterns that vary systematically across neural systems. This early work established a critical principle: brain charts are not a single curve, but a family of trajectories across multiple phenotypes, each with its own maturational chronology. The consolidation of brain chart methodology reached a milestone with the aggregation of 123,984 MRI scans from over 100 primary studies, spanning 115 days post-conception to 100 years of age (6). This effort extended the previous methodological demonstration into a highly usable resource by producing the first comprehensive normative growth curves for multiple global and regional brain morphometric phenotypes with GAMLSS. These charts achieved several key advances (Fig. 1c):
- (1)
- Centile scores translate population-level normative channels into precise coordinates for each individual brain, thereby quantifying where any brain sits within Waddington's "valley", transforming abstract developmental stability into a measurable distance.
- (2)
- Neurodevelopmental milestones delineate the "contour lines" of the developmental landscape, revealing spatiotemporal nodes where the slope (growth velocity) and topography (tissue volume) of the canalized channel change most abruptly, providing empirical yardsticks for understanding sensitive periods.
- (3)
- By tracking individual centile shifts over time, we can quantify the rate at which a person traverses the landscape, i.e., the dynamic process of deviating from or returning to the population channel, thereby upgrading Waddington's canalization from a static cross-section to a kinetic description with velocity and acceleration.
- (4)
- Centile deviations in clinical cohorts, together with enhanced heritability, jointly anchor the biological bottom line of landscape deviation, indicating that the "depth" (variability) of the valley possesses a specific genetic architecture, and providing a biological basis for defining risk thresholds beyond which a trajectory departs from typical neurodevelopment.
From a landscape perspective, the brain chart is an empirical instantiation of Waddington’s valley: the centile curves trace the boundaries of the developmentally accessible channel, while the dispersion of individual centile scores captures the width and depth of the canalized path at each age. The finding that variability itself changes over time, increasing in gray matter during infancy, peaking in subcortical structures during adolescence, and rising sharply in ventricles during ageing, reveals that the canalized channel is not of uniform width; it widens or narrows across developmental epochs, reflecting changing constraints and opportunities for plasticity.
Despite its utility, the biological validity of brain charts has faced persistent challenges. Brain charts are primarily derived from structural MRI phenotypes, whose cellular and molecular underpinnings are only partially understood. A low centile score for cortical thickness does not inherently inform the clinician or scientist about the underlying biological processes, whether it reflects reduced synaptic density, altered myelination, shifts in dendritic arborization, or simply the influence of head size. This ambiguity limits the translational power of brain charts, as the same centile deviation could arise from vastly different causal mechanisms. Within the brainality landscape framework, this biological validity challenge can be substantially addressed through multiscale cross-validation. By embedding brain charts within the three-dimensional coordinate system of the landscape, gradients, lifespan, and individual neural differentiation, we can interrogate the biological meaning of centile deviations in a principled manner.
- (1)
- Linking centile deviation to gradient dimensions: A child with low centile scores in the SA gradient might show delayed maturation of association cortex, whereas low centile scores in the visual-somatosensory axis might reflect modality-specific differences. By mapping centile deviations onto gradient topographies, we can distinguish local from global atypicalities and link them to known molecular or functional axes.
- (2)
- Connecting centile trajectories to gene expression and cellular profiles: Using transcriptomic atlases and virtual histology, we can ask which genes or cell types are enriched in brain regions where centile deviations are most pronounced. This allows us to move from descriptive centile scores to mechanistic hypotheses, e.g., that early life reduction in gray matter centiles is associated with synaptic signaling genes, or that late-life centile decline in white matter tracks myelination-related transcripts.
- (3)
- Validating centile predictions with functional and behavioural measures: The same individuals whose brain structure falls at a given centile can be assessed for cognitive performance, psychiatric symptoms, or real-world outcomes. This establishes a direct link between normative structural benchmarks and functional relevance.
In practice, this multiscale approach turns brain charts into a richer instrument: a given centile score is no longer a standalone number but is interpreted in the context of gradient position, developmental stage, and available multimodal evidence. For example, an adolescent whose subcortical gray matter volume lies at the 5th centile, whose SA gradient is within normal range, and whose amygdala-centile deviation aligns with expression of serotonergic genes, might be interpreted very differently from a similar centile deviation in a different gradient context. Ultimately, brain charts serve as the operational link between the macroscopic laws of neurodevelopment and the idiosyncratic trajectories of individual lives. They transform Waddington’s landscape from a qualitative metaphor into a quantitative, empirically grounded reference system. The lifespan dimension anchors each individual in developmental time; the centile dimension situates each individual relative to the population channel; and the gradient dimension adds spatial and biological specificity. The road ahead lies in refining these charts with greater demographic diversity, extending them to multimodal phenotypes (functional connectivity, diffusion metrics, perfusion), and integrating them with longitudinal tracking to capture dynamic changes within individuals. The brainality landscape framework provides the conceptual and analytical scaffolding to interpret brain chart deviations not as isolated anomalies but as signals that arise from the interplay of molecular gradients, developmental timing, and individual experience, a true multiscale integration that enhances biological validity and accelerates clinical translation.
Toward a Unified Biophysical Framework
The brainality landscape, defined by three orthogonal dimensions: gradients (space), lifespan (time), and individual neural differentiation (variation), provides a conceptual scaffold for integrating phenomena across multiple scales. To transform this conceptual scaffold into a predictive, quantitative framework, we must formalize it using the mathematics of stochastic dynamical systems (see Box 1). Here we draw on approaches developed in statistical mechanics and systems biology (26) to model neurodevelopment as a stochastic process evolving on a complex landscape. Let the state of a developing brain at time t be described by a high-dimensional vector x(t) representing, for example, the position of an individual along the three dimensions of the brainality landscape. In the spirit of Waddington's canalization, the dynamics of x(t) are governed by both deterministic forces (the shape of the landscape, reflecting genetic and epigenetic constraints) and stochastic fluctuations (arising from molecular noise, environmental variability, and individual experience).
We propose the following Langevin equation as a general model for neurodevelopmental dynamics:
where:
- (1)
- U(x;θ(t)) is the quasipotential landscape that defines the attractor states of the system. This landscape is parameterized by θ(t), a set of time-dependent parameters that capture the lifespan dimension, the fact that the landscape itself changes over developmental time.
- (2)
- −∇U is the deterministic force that pushes the system toward local minima (attractors) of the landscape, corresponding to canalized developmental outcomes.
- (3)
- η(t) is a stochastic noise term, representing intrinsic and extrinsic sources of variability that drive individual neural differentiation.
Crucially, the quasipotential U is not directly observable but can be inferred from the probability distribution of states P(x) using the Boltzmann-Gibbs relation:
U(x)∝lnP(x)
This relationship provides a direct link between empirically measured distributions (e.g., brain charts, gradient atlases) and the underlying landscape. The ultimate goal of the brainality landscape framework is to predict how perturbations, genetic variants, early adversity, educational interventions, socioeconomic status, shift an individual's trajectory within the landscape. For a given perturbation ∆θ(t) (a change in the parameters that define the landscape, or the parameter space of the landscape), we can compute the resulting shift in the probability distribution of states using linear response theory:
This equation formalizes the essence of a Pinball Life Machine. In this metaphor (Fig. 1d), the perturbation ∆θ represents the player's action, pressing a flipper, adjusting a bumper, or introducing a targeted environmental change, while the resulting shift ∆P captures the altered odds of landing in a particular developmental outcome. Without quantitative modeling, such actions are guesses; with it, they become informed interventions whose effects on the entire distribution of developmental trajectories can be forecast. Just as a skilled pinball player learns the machine's physics to redirect the ball, quantitative landscape modeling allows us to predict which perturbations at which critical windows will most effectively steer an individual's trajectory away from maladaptive attractors and toward healthier basins of attraction. This shift from qualitative description to quantifiable prediction is precisely what transforms the brainality landscape from a compelling metaphor into a rigorous, testable framework for precision life management. This allows us to predict, for example, how a specific genetic variant that affects synaptic pruning might shift the trajectory of the SA gradient, or how an early educational intervention might increase the fidelity of the SA gradient to the canonical template and thereby enhance cognitive outcomes.
NeuroAI Acceleration for Shaping Brainality Landscape
Artificial intelligence (AI) can contribute to the brainality landscape at four interconnected levels. First, at the level of data organization, large language models and agentic AI systems can automate metadata annotation, literature screening, data-dictionary alignment, quality control, and preprocessing orchestration across heterogeneous cohorts. This is not a marginal efficiency gain: population neuroscience is chronically constrained by labor-intensive curation, and automated governance-aware pipelines can compress months of harmonization into days while improving auditability. Second, at the level of representation learning, AI can extract low-dimensional gradient coordinates from high-dimensional connectomes and multimodal phenotypes, providing empirically grounded embeddings for the state vector x(t). Foundation models of neural activity, brainnets, and behavior can further improve prediction of individual developmental stage and deviation from normative channels. Third, at the level of mechanistic inference, AI can help solve the inverse problem at the heart of the framework: estimating P(x | age) from brain charts, constraining low-dimensional coordinates with gradient atlases, inferring the drift term −∇U and noise amplitude η(t) from longitudinal trajectories, and fitting stochastic differential equations through simulation-based inference and Bayesian inversion. Fourth, at the level of perturbation prediction, causal machine learning, digital twins, and reinforcement learning can approximate the linear response, allowing candidate "flipper actions", educational, clinical, or community interventions, to be evaluated in silico before empirical deployment, and allowing sensitive windows to be identified with greater precision.
The above AI acceleration must remain theory-constrained rather than becoming a new form of black-box curve-fitting. The optimization framework articulated by Richards and colleagues (27) including objective functions, learning rules, and architectures, offers a principled template: AI models for the brainality landscape should be constrained by developmental priors, synaptic plasticity rules, hierarchical architectures, and biological plausibility, and should be evaluated not only by predictive accuracy but by mechanistic interpretability. As Sadeh and Clopath (28) emphasize, a model that perfectly predicts neural activity without providing mechanistic insight offers limited scientific value. In the brainality context, the standard must be even higher: AI must help estimate the landscape, not merely interpolate the data.
The empirical realization of the brainality landscape depends on data that are simultaneously large-scale, lifespan-spanning, demographically diverse, multimodal, and longitudinally tracked. Current flagship cohorts and their brain-chart derivatives have been monumental, but they remain individual monuments rather than parts of a connected city (29). Data are siloed within institutions and consortia, acquired with heterogeneous protocols, and governed by complex access agreements that often stifle collaboration before it begins. The BrainNet vision addresses this fragmentation through four pillars: global scale and diversity across the lifespan; standardization and interoperability; open science by design with tiered access and federated analysis; and a living benchmark for NeuroAI. For the brainality landscape, each pillar maps directly onto a modeling requirement. Global diversity is necessary because brain charts built on narrow demographic slices are inherently biased and clinically inadequate for global application; standardization is necessary because gradients and centile trajectories can only be pooled if phenotypes are harmonized; open science by design is necessary because the quasipotential landscape must be estimated from distributions, not from a handful of convenience samples; and a living NeuroAI benchmark is necessary because the framework's ultimate test is predictive generalization to new individuals, cohorts, and contexts.
The technical architecture already exists in prototype. Federated learning allows models to be trained across distributed datasets without centralizing raw data; algorithms can be sent to the data rather than data to the algorithms. Trusted research environments and federated analysis frameworks provide concrete mechanisms for cross-site computation under restrictive legal regimes. What BrainNet adds is a common normative target: a globally harmonized, lifespan-spanning reference system for brain charts, gradient manifolds, and individual deviation metrics (BrainNetTypes) that can serve as the empirical substrate for landscape estimation and as the benchmark against which brain-inspired AI is evaluated. The BrainNet imperative cannot be realized without confronting a fundamental tension that Ray and colleagues articulate with unusual clarity (30): the open science movement and the tightening of data sovereignty regimes are pulling in opposite directions. Governments increasingly treat data as national assets subject to legal, economic, and geopolitical controls. These constraints are not merely bureaucratic obstacles. They reflect a deeper reconceptualization of neural data. Unlike genetic or proteomic data, many forms of neural data capture dynamic patterns of activity that reflect attention, valuation, emotion, and decision-making, and when integrated with behavioral, linguistic, and physiological measures, they can support inference of latent mental states. Neural data therefore occupy a distinctive position in relation to personhood and require stratified, modality-specific governance rather than treatment as a homogeneous category of health data. Moreover, value increasingly resides not only in raw data but in derived models trained on those data: models that can encode individual-level patterns with high predictive fidelity and that may be deployed across jurisdictions in ways that existing privacy frameworks do not adequately govern.
The central empirical objects of brainality landscape (brain charts, gradient atlases, centile trajectories, and landscape parameters) are derived representations, not raw data. If governance remains focused exclusively on data transfer while ignoring derived models, then the most scientifically and commercially valuable outputs of population neuroscience will escape oversight. Conversely, if governance becomes so restrictive that cross-border collaboration collapses, the landscape will be estimated from unrepresentative samples, and its clinical and policy relevance will be correspondingly limited. The framework therefore requires a governance model that is simultaneously enabling and protective: one that recognizes neural data as both a scientific resource and a strategic asset, and that extends oversight from raw data to derived computational representations. A set of operational international data governance instruments that are directly relevant to the brainality landscape has been proposed recently (29,30). They constitute what we would call governance infrastructure for the landscape: they translate legal and ethical requirements into machine-actionable metadata and reusable institutional competencies, reducing the friction that currently prevents pooled analysis across jurisdictions.
For population neuroscience, the lesson is that governance should be treated as an enabler of discovery, a precondition for the large-scale, diverse, and longitudinally tracked datasets that the brainality landscape requires, rather than as an external constraint to be minimized. It explicitly includes culture, community, country, and region among the factors that shape developmental trajectories. This inclusion carries a governance implication that is often overlooked: cultural context is not noise to be averaged away, but a parameter of the landscape that must be represented in the data and in the models. If global brain charts are built predominantly from high-income, Western, educated, industrialized, rich, and democratic samples, then the normative channels they define will encode the developmental trajectories of a narrow slice of humanity and will misclassify individuals from other contexts as deviant. The consequences are not merely scientific but ethical: brain-based predictions and interventions calibrated on unrepresentative norms can pathologize difference and exacerbate inequalities. Ray and colleagues describe the risk of "data colonialism", the extraction of data from marginalized communities with limited local involvement or lasting benefit, and the related phenomenon of "parachute science." These risks are particularly acute in population neuroscience, where large cohorts in low- and middle-income countries may be attractive to external researchers precisely because they offer diversity, yet may lack the infrastructure, training, and governance capacity to ensure that benefits are shared. The brainality landscape framework cannot afford this extractive model. Its validity depends on diverse and representative data, and its legitimacy depends on equitable collaboration. Benefit-sharing templates, local analytic access, capacity building, and governance participation are therefore not optional add-ons; they are conditions for the scientific success of the framework.
A related challenge is the risk of pseudo-scientific inference. As Birhane warns (31), the use of inscrutable AI tools to infer inner attributes from brain or body data can lend a veneer of objectivity to outdated and harmful claims. In the context of the brainality landscape, the danger is that centile deviations and gradient positions could be reified into deterministic predictions about individuals, predictions that ignore context, measurement error, and the fundamentally probabilistic nature of developmental trajectories. The framework's own mathematics cautions against this: the landscape is stochastic, the noise term η(t) is irreducible, and the quasipotential is inferred from population distributions rather than read directly from any individual brain. Governance must therefore include not only privacy protection but epistemic humility against individual-level deterministic interpretation.
Bringing these strands together, we propose that the brainality landscape be operationalized through a federated, governance-aware research architecture with five components. First, a harmonized data layer: BrainNet-style (29) interoperable datasets adhering to standard principles, formats, and machine-readable governance labels, spanning the lifespan and representing global diversity. Second, a federated analytics layer: trusted research environments and federated learning frameworks that allow models to be trained and validated across jurisdictions without centralizing raw data, with algorithms sent to the data and only model parameters or summary statistics returned. Third, a model governance layer: derived-model registries, provenance tracking, inference-risk assessment, and continuous audit, ensuring that the landscape parameters and predictive models themselves are governed as scientific outputs. Fourth, a coordination layer: an international data governance body, building one that maintains legal guides, governance templates, accreditation mechanisms, and rapid-response sandboxes, and that represents neuroscience in geopolitical discussions of data access and sovereignty. Fifth, a capacity-building layer: training, infrastructure, and equitable partnership mechanisms that enable institutions to participate fully in data generation, analysis, and governance, thereby avoiding data colonialism and improving the representativeness of the landscape. This architecture directly serves the scientific goals of the brainality landscape. The harmonized data layer provides the empirical distributions from which the quasipotential is inferred. The federated analytics layer allows the inverse problem to be solved across diverse cohorts without violating sovereignty constraints. The model governance layer ensures that the resulting landscape parameters and predictive models are transparent, auditable, and responsibly deployed. The coordination layer reduces the transaction costs that currently prevent cross-border collaboration. The capacity-building layer expands the empirical base and enhances the generalizability of the framework.
Several challenges must be confronted honestly. First, big data are not the same as high-quality data: automated annotation and agentic pipelines can amplify batch effects, missingness mechanisms, and cultural biases unless accompanied by rigorous quality control, provenance tracking, and external validation. Second, prediction is not mechanism: a high-performing model that cannot explain why a centile deviation arises offers limited translational value, and the brainality framework must therefore prioritize models that link centile deviations to gradient positions, gene expression, cellular profiles, and functional outcomes. Third, causal inference from observational cohorts remains difficult: AI-based association analyses are vulnerable to spurious correlations, and the framework's perturbation predictions must be validated through longitudinal designs, natural experiments, and intervention trials rather than accepted on the basis of model fit alone. Fourth, privacy and governance are not optional: the framework must operate within existing legal frameworks, and its global ambitions must not become an excuse for circumventing consent, sovereignty, or equity. Fifth, there is a risk of over-reliance on computational tools at the expense of biological insight and analytical rigor; the field must not create a generation of researchers who can execute sophisticated pipelines but cannot critically evaluate their results. These challenges argue for a balanced approach: AI should be used to accelerate the loop from data to model to perturbation to validation, but the loop must remain anchored in biological theory, governed by transparent and equitable rules, and evaluated by criteria that include mechanistic insight, reproducibility, and real-world benefit. The brainality landscape's mathematical structure (stochastic dynamics, quasipotential inference, linear response) provides a natural framework for this balance on taking a shape of the epibrainnetics, because it forces every AI-derived prediction to be expressed as a statement about landscape parameters, noise, or perturbation response, rather than as an uninterpretable black-box output.
The convergence of AI, open science, and international data governance creates a rare window of opportunity for population neuroscience. In the data layer, AI can compress years of curation into months and maintain dynamic, governance-aware data catalogs. In the modeling layer, foundation models, neural stochastic differential equations, and simulation-based inference can integrate brain charts, gradient atlases, and longitudinal trajectories into an updatable landscape atlas, moving the field from descriptive curve-fitting to perturbation prediction. In the validation layer, digital twins and virtual trials can screen candidate interventions before real-world deployment, reducing the cost and ethical burden of large-scale trials. In the globalization layer, federated learning and local calibration can allow ABCD (32), CCBD (33), and other cohorts to complement one another, increasing sample diversity while preserving cultural specificity. In the governance layer, instruments such as machine-readable governance labels, derived-model registries, cross-border accreditation, and benefit-sharing templates can reduce the friction that currently prevents global collaboration, while safeguarding the rights and interests of participants and jurisdictions. The ultimate measure of success is not the sophistication of the AI tools or the size of the datasets, but whether the field can generate mechanistic insight and actionable prediction at a global scale. The brainality landscape provides the theoretical scaffold; BrainNet provides the data and benchmarking infrastructure; federated analytics provides the technical means; and international data governance provides the legal and ethical framework. Together, these elements can transform population neuroscience from a collection of isolated cohorts and descriptive charts into a coordinated, predictive, and equitable science, one capable of estimating the landscape of human brain development with sufficient precision to guide interventions, and with sufficient humility to respect the irreducible variability of individual lives.
Conclusion
The brainality landscape framework, formalized through stochastic differential equations and grounded in the mathematics of quasipotential landscapes and enabled by a federated, governance-aware AI ecosystem, provides a biophysical and operational scaffold for Developmental Population Neuroscience. By linking the three dimensions of the landscape, gradients, lifespan, and individual differentiation, to quantitative models of attractor dynamics, entropy, and response to perturbations, this framework transforms the landscape from a metaphor into a predictive, testable model. The application to Pinball Life Machine illustrates how the framework can accommodate both trait-like (topological) and state-like (connectivity) features of brain disorders, and suggests new directions for intervention: targeting the landscape itself (e.g., by reshaping attractors) rather than merely treating symptoms. As we continue to populate this framework with mechanistic models and empirical data (34-37) (see Box 2), we move closer to a mature, predictive science of human neurodevelopment, one that can guide not only our understanding but also our ability to steer individual brains toward healthier paths.
Box 1: Stochastic Differential Equations - A quantitative language for the brainality landscape
Biological development is inherently stochastic. At the molecular level, gene expression fluctuates; at the circuit level, neural activity is noisy; and at the environmental level, experience is variable. To capture these dynamics in a quantitative framework, we turn to stochastic differential equations (SDEs), a mathematical formalism that combines deterministic forces with random fluctuations. SDEs describe how the state of a system, such as an individual’s position on the brainality landscape, evolves over time under the influence of both predictable (canalized) and unpredictable (noise) influences. The Boltzmann-Gibbs equation provides the empirical bridge between large-scale neuroimaging data and the landscape. If we can estimate the probability that an individual at a given age occupies a particular position in the landscape, we can reconstruct the underlying landscape topography. Regions of high probability correspond to deep attractors; regions of low probability correspond to barriers or rarely visited states.
How do we estimate the probability and the landscape parameters from real data? The answer lies in the convergence of three pillars of Developmental Population Neuroscience: 1) brain charts provide the empirical distributions of structural and functional brain phenotypes across age. By quantifying centile scores for multiple phenotypes (e.g., gray matter volume, cortical thickness, surface area, diffusion metrics), we obtain a joint probability distribution P(x(t)|age), the likelihood of observing a given brain state at a given developmental stage. 2) Gradients offer a low-dimensional embedding of cortical organization, providing a natural coordinate system for x, reducing the high-dimensional brain state space to a manageable set of continuous dimensions that capture the dominant modes of variation. The normative trajectory of these gradients across the lifespan, as well as their inter-individual variability, directly informs the time-dependent parameters. 3) Longitudinal tracking of individuals over time provides the dynamic data needed to estimate not only the stationary distribution, but also transition probabilities between states. The rate at which an individual’s centile scores change (velocity) and the acceleration of those changes reveal the local slope of the landscape and the strength of the restoring force toward the canalized channel.
Integrating these three sources, we can fit the landscape parameters at each age by: 1) Estimating the empirical distribution from cross-sectional brain chart data; 2) Extracting the dominant gradient coordinates; 3) Modeling the longitudinal trajectories to infer the deterministic drift and the noise amplitude. Mathematically, this is equivalent to solving the inverse problem: given observed trajectories, find the landscape and noise that best reproduce the data. This can be achieved through maximum likelihood estimation or Bayesian inference. This SDE framework, grounded in empirical brain charts and gradient atlases, provides a principled way to: 1) Identify critical periods when the landscape is most sensitive to perturbations; 2) Simulate the effects of specific interventions on individual trajectories; 3) Quantify the risk of deviation from typical development for a given individual; 4) Design personalized “flipper actions” that steer the trajectory toward healthier basins.
By bridging the gap between descriptive growth curves and predictive dynamical models, the brainality landscape moves beyond metaphor, it becomes a testable, data-driven, and mathematically grounded framework for precision life management in developmental neuroscience.
Box 2. Population neuroscience resources for the Brainality Landscape modeling
In 2016, the National Institutes of Health in the United States initiated the Adolescent Brain Cognitive Development (ABCD) study (32). The ABCD study is a large longitudinal cohort study of 11,880 children and their parents that is currently continuing data collection at research sites in 21 metropolitan areas of the United States. The baseline ABCD sample was ethnically diverse by design (51% White, 21.4% Hispanic, 15.2% African American, 2.3% Asian, 10.01% multiracial/other). The full sample includes siblings as well as twins. Children are followed annually for 10 years starting at approximately 9-10 years of age. The baseline visit consisted of clinical interviews, surveys, neurocognitive tests, biospecimens, and neuroimaging. Subsequent data collection timepoints alternate between on-line assessments and in-lab assessments with full cognitive and neuroimaging data collection. Over 2000 publications have already resulted from this large population neuroscience dataset, which continues to be used by researchers worldwide to answer questions relevant to youth mental health, substance use, and brain development (38).
In 2021, the China Brain Project (CBP, 39) initiated the Chinese Child Brain Development (CCBD) study (33). The CCBD study aims to investigate the environmental and genetic factors that affect brain and cognitive development, academic performance, and psychological well-being. A cross-sectional sample of more than 5,000 participants aged 6-18 years has been collected during the first five years. The CCBD study contains a large longitudinal cohort of more than 26,000 children aged 6-7 years, who will be followed annually until they are 18 years old. The CCBD study also includes a prospective cohort that follows 10,000 children aged 3-8 years to investigate the causes of Chinese dyslexia, and the extension cohort from the existing Born in Guangzhou Cohort Study (40) to follow up 10,000 children aged 6-12 years for investigating the early predictors of learning difficulties and mental health problems. Extensive cognitive and behavioural, socioemotional, environmental, EEG, neural and genetic data have been collected for the CCBD baseline visits and ongoing for the follow-up visits. Combined with existing big data resource such as the ABCD study, the CCBD study will expand the scope of questions that can be explored through the brainality landscape framework. With these big data of Developmental Population Neuroscience, the CCBD study expects to substantially improve the reliability and generalizability of scientific discovery.
Author Contributions
XNZ drafted the manuscript and revised it with LQU.
Funding
The Brain Science and Brain-like Intelligence Technology-National Science and Technology Major Project grant 2021ZD0200500 (XNZ). The National Institute of Child Health and Human Development grant R21HD111805 and R01HD11669 (LQU).
Acknowledgments
The intellectual journey that has culminated in this Perspective spans more than a decade of interdisciplinary collaboration, sustained institutional support, and countless conversations across laboratories, conferences, and classrooms. It is a privilege to express our gratitude to the many individuals and organizations whose contributions have shaped Developmental Population Neuroscience into the vibrant field it is today. The International Conference on Human Brain Development (ICHBD, https://www.brain-net.cn/ichbd2026) has been the foundational engine of this enterprise. Over the past twelve years, seven ICHBD meetings have brought together developmental neuroscientists, geneticists, epidemiologists, clinicians, methodologists, and computational scientists from around the world. These conferences were not merely venues for presenting results; they were incubators of ideas, crucibles of cross-disciplinary synthesis, and the social fabric from which Developmental Population Neuroscience emerged. We thank the Chinese Academy of Sciences (CAS) and the CAS Institute of Psychology for hosting and supporting multiple ICHBD meetings, and the Beijing Normal University for its unwavering commitment to advancing brain science through international dialogue. The spirit of openness, rigor, and collegiality that has characterized ICHBD from its first meeting in 2014 to its most recent gathering is the very spirit that has propelled this field forward. The scientific foundation of Developmental Population Neuroscience rests on large-scale, population-based neuroimaging cohorts. We are deeply grateful to all members of the Chinese Color Nest Project (CCNP) and its successors, the CCBD (Chinese Child Brain Development) and DLPFC (Decade circLe CCNP Family Cohort) studies, whose collective efforts have transformed the vision of developmental brain mapping into a tangible, longitudinal reality. We thank the investigators, research coordinators, data managers, MRI technologists, and administrative staff at the Beijing Normal University, the CAS Institute of Psychology, the Science Data Bank (https://brain-net.cn/ccndc), and our partner institutions for their tireless dedication. Their meticulous work has made it possible to chart the brain's developmental landscape with unprecedented precision. We are equally indebted to the broader international consortia that have shaped the conceptual and empirical infrastructure of the field, including the Adolescent Brain Cognitive Development (ABCD) Study, the Functional/Human Connectome Project (FCP/HCP), and the UK Biobank. These initiatives have demonstrated that large-scale data sharing and collaborative harmonization are not merely aspirational ideals but achievable realities. They have provided normative reference data, empirical maps, that underpin brain charts and gradient atlases. We thank the principal investigators, funding agencies, and participating scientists who have championed open science and built the infrastructure that enables population neuroscience to flourish. Finally, and most personally, we thank the students of our courses on Developmental Cognitive Neuroscience and Developmental Population Neuroscience across all levels, from undergraduate and graduate students to postdoctoral fellows and visiting scholars. Teaching is often described as a one-way transmission of knowledge, but our experience has been quite the opposite: it is a dialogue, a shared exploration, and a constant source of renewal. The classroom has been a laboratory of ideas, where the abstractions of landscapes, gradients, and charts are tested against the lived realities of human development. Your energy and curiosity have been the catalyst that keeps us engaged, humble, and excited about the future of this discipline. We also acknowledge the families and children who have participated in our longitudinal studies. Your trust and generosity, sharing your time, your brains, and your stories, are the real foundation of Developmental Population Neuroscience. As we submit this Perspective, we are mindful that the landscape we describe is itself a work in progress. It will be reshaped by the next generation of students, the next wave of data, and the next iteration of ICHBD. We look forward to that unfolding with anticipation and hope.
Competing interests
Authors declare that they have no competing interests.
References
- Paus, T. Population neuroscience: why and how. Hum. Brain Mapp. 2010, 31, 891–903. [Google Scholar] [CrossRef]
- Zuo, X.N.; He, Y.; Su, X.; Hou, X.H.; Weng, X.; Li, Q. Developmental population neuroscience: emerging from ICHBD. Sci. Bull. 2018, 63, 331–332. [Google Scholar] [CrossRef]
- Falk, E.B.; et al. What is a representative brain? Neuroscience meets population science. Proc. Natl. Acad. Sci. U. S. A. 2013, 110, 17615–176122. [Google Scholar] [CrossRef]
- Paus, T. Population neuroscience: Principles and advances. Curr. Top. Behav. Neurosci. 2024, 68, 3–34. [Google Scholar] [CrossRef]
- Waddington, C.H. Canalization of development and the inheritance of acquired characters. Nature 1942, 150, 563–565. [Google Scholar] [CrossRef]
- Bethlehem, R.A.I.; et al. , Brain charts for the human lifespan. Nature 2022, 604, 525–533. [Google Scholar] [CrossRef]
- Biswal, B.B.; Yetkin, F.Z.; Haughton, V.M.; Hyde, J.S. Functional connectivity in the motor cortex of resting human brain using echo-planar MRI. Magn. Reson. Med. 1995, 34, 537–541. [Google Scholar] [CrossRef]
- Biswal, B.B.; Uddin, L.Q. The history and future of resting-state functional magnetic resonance imaging. Nature 2025, 641, 1121–1131. [Google Scholar] [CrossRef]
- Vincent, J.L.; et al. , Intrinsic functional architecture in the anaesthetized monkey brain. Nature 2017, 447, 83–86. [Google Scholar] [CrossRef]
- Yeo, B.T.T.; et al. , The organization of the human cerebral cortex estimated by intrinsic functional connectivity. J. Neurophysiol. 2011, 106, 2322–2345. [Google Scholar] [CrossRef]
- Uddin, L.Q. Salience processing and insular cortical function and dysfunction. Nat. Rev. Neurosci. 2015, 16, 55–61. [Google Scholar] [CrossRef]
- Smith, S.M.; et al. Correspondence of the brain's functional architecture during activation and rest. Proc. Natl. Acad. Sci. U. S. A. 2009, 106, 13040–13045. [Google Scholar] [CrossRef]
- Kong, R.; et al. , A network correspondence toolbox for quantitative evaluation of novel neuroimaging results. Nat. Comms. 2025, 16, 2930. [Google Scholar] [CrossRef]
- Dubois, J.; Adolphs, R. Building a science of individual differences from fMRI. Trends Cogn. Sci. 2016, 20, 425–443. [Google Scholar] [CrossRef]
- Finn, E.S.; et al. , Functional connectome fingerprinting: identifying individuals using patterns of brain connectivity. Nat. Neurosci. 2015, 18, 1664–1671. [Google Scholar] [CrossRef]
- Margulies, D.S.; et al. , Situating the default-mode network along a principal gradient of macroscale cortical organization. Proc. Natl. Acad. Sci. U. S. A. 2016, 113, 12574–12579. [Google Scholar] [CrossRef]
- Huntenburg, J.M.; Bazin, P.L.; Margulies, D.S. Large-scale gradients in human cortical organization. Trends Cogn. Sci. 2018, 22, 21–31. [Google Scholar] [CrossRef]
- Huang, Z.; et al. An opposing molecular gradient axis underlies primate cortical organization. Science 2026, 392, eaea2673. [Google Scholar] [CrossRef]
- Tsyporin, J.; et al. Competing programs shape cortical sensorimotor–association axis development. Nature 2026, 656, 688–699. [Google Scholar] [CrossRef]
- Taylor, H.P.; et al. Functional hierarchy of the human neocortex across the lifespan. Nature 2026, 652, 955–964. [Google Scholar] [CrossRef]
- Dong, H.M.; Margulies, D.S.; Zuo, X.N.; Holmes, A.J. Shifting gradients of macroscale cortical organization mark the transition from childhood to adolescence. Proc. Natl. Acad. Sci. USA 2021, 118, e2024448118. [Google Scholar] [CrossRef]
- Sydnor, V.J.; et al. , Neurodevelopment of the association cortices: patterns, mechanisms, and implications for psychopathology. Neuron 2021, 109, 2820–2846. [Google Scholar] [CrossRef]
- Sydnor, V.J.; et al. Intrinsic activity development unfolds along a sensorimotor–association cortical axis in youth. Nat. Neurosci. 2023, 26, 638–649. [Google Scholar] [CrossRef]
- Chen, L.Z.; Holmes, A.J.; Zuo, X.N.; Dong, Q. Neuroimaging brain growth charts: A road to mental health. Psychoradiology 2021, 1, 272–286. [Google Scholar] [CrossRef]
- Xu, T.; Yang, Z.; Jiang, L.; Xing, X.X.; Zuo, X.N. A Connectome Computation System for discovery science of brain. Sci. Bull. 2015, 60, 86–95. [Google Scholar] [CrossRef]
- Feinberg, A.P.; Levchenko, A. Epigenetics as a mediator of plasticity in cancer. Science 2023, 379, eaaw3835. [Google Scholar] [CrossRef]
- Richard, B.A.; et al. , A deep learning framework for neuroscience. Nat. Neurosci. 2019, 22, 1761–1770. [Google Scholar] [CrossRef]
- Sadeh, S.; Clopath, C. The emergence of NeuroAI: bridging neuroscience and artificial intelligence. Nat. Rev. Neurosci. 2025, 26, 583–584. [Google Scholar] [CrossRef]
- Zuo, X.N. The BrainNet imperative: why global brain science needs its own ImageNet moment. Sci. Bull. 2026, 71, 1587–1590. [Google Scholar] [CrossRef]
- Ray, K.L.; et al. Reconciling global collaboration and data sovereignty in neuroscience. Nat. Neurosci. 2026, 29, 2397–2407. [Google Scholar] [CrossRef]
- Witten, et al. Future views on neuroscience and AI. Cell 2024, 187, 5809–5813. [Google Scholar] [CrossRef]
- Barch, D.M.; et al. , Demographic and mental health assessments in the adolescent brain and cognitive development study: Updates and age-related trajectories. Dev. Cogn. Neurosci. 2021, 52, 101031. [Google Scholar] [CrossRef]
- Liu, N. Landscaping neurodevelopment of attention-deficit hyperactivity disorder. Sci. Bull. 2026, 71, 5058–5072. [Google Scholar] [CrossRef]
- Pang, J.C.; et al. , Geometric constraints on human brain function. Nature 2023, 618, 566–574. [Google Scholar] [CrossRef]
- Normand, F.; et al. Geometric constraints on the architecture of mammalian cortical connectomes. Cell 2026, 189, 5283–5303.e17. [Google Scholar] [CrossRef]
- Marek, S.; et al. Patterns of brain-wide associations reflect socioeconomics. Science 2026, 392, eaee6213. [Google Scholar] [CrossRef]
- Yücel, A.D.; Molière, A.; Gladyshev, V.N. Written in development and lost in ageing: the grammar of cellular identity. Nature 2026, 658, 45–54. [Google Scholar] [CrossRef]
- Karcher, N.R.; Barch, D. M. The ABCD study: understanding the development of risk for mental and physical health outcomes. Neuropsychopharmacology 2021, 46, 131–142. [Google Scholar] [CrossRef]
- Liu, X.; Gao, T.; Lu, T.; Bao, Y.; Schumann, G.; Lu, L. China Brain Project: from bench to bedside. Sci. Bull. 2023, 68, 444–447. [Google Scholar] [CrossRef]
- Huang, S.; et al. The Born in Guangzhou Cohort Study enables generational genetic discoveries. Nature 2024, 626, 565–573. [Google Scholar] [CrossRef]
Figure 1.
The brainality landscape for developmental population neuroscience. A) The brainality landscape is revised from Waddington’s landscape in epigenetics. The colorful ball represents a topological equivalent of the human brain. The color indicates functional hierarchy. This landscape contains three dimensions including gradients, lifespan and individual neural differentiation. B) Gradient mapping on brain surface and its topologically transformed sphere. This sensorimotor (blue)-association (yellow) map is from the seminal gradient work (16). C) Human brain charts characterize the group-level development trajectories and individual differentiation of the white matter volumes at different levels (from 2% to 98%). These data are from the seminal chart work (6). Multiple occasions of individual records from the same person are plotted on the normative chart graph with arrows indicating the individual developmental curve. D) A pinball life machinery is visualized for developmental population neuroscience (DevPopNeurosci). It summarizes various factors to modify the trajectories on the landscape by using vivo or in-vivo approaches. The factors cover from micro- to macro-scales including cell, individual (IDV), personal networks (PSN), community (CMY), country and region (CTR), culture (CUR). Each scale contains many different factors, which are documented with details in (3). Several slingshots are set to highlight the key variables for changing the ball’s trajectories: the patient model (PAT), sports (SPT), education (EDU) and socioeconomic status (SES). E) The Adolescent Brain Cognitive Development (ABCD) study. F) The Chinese Child Brain Development (CCBD) study.
Figure 1.
The brainality landscape for developmental population neuroscience. A) The brainality landscape is revised from Waddington’s landscape in epigenetics. The colorful ball represents a topological equivalent of the human brain. The color indicates functional hierarchy. This landscape contains three dimensions including gradients, lifespan and individual neural differentiation. B) Gradient mapping on brain surface and its topologically transformed sphere. This sensorimotor (blue)-association (yellow) map is from the seminal gradient work (16). C) Human brain charts characterize the group-level development trajectories and individual differentiation of the white matter volumes at different levels (from 2% to 98%). These data are from the seminal chart work (6). Multiple occasions of individual records from the same person are plotted on the normative chart graph with arrows indicating the individual developmental curve. D) A pinball life machinery is visualized for developmental population neuroscience (DevPopNeurosci). It summarizes various factors to modify the trajectories on the landscape by using vivo or in-vivo approaches. The factors cover from micro- to macro-scales including cell, individual (IDV), personal networks (PSN), community (CMY), country and region (CTR), culture (CUR). Each scale contains many different factors, which are documented with details in (3). Several slingshots are set to highlight the key variables for changing the ball’s trajectories: the patient model (PAT), sports (SPT), education (EDU) and socioeconomic status (SES). E) The Adolescent Brain Cognitive Development (ABCD) study. F) The Chinese Child Brain Development (CCBD) study.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (http://creativecommons.org/licenses/by/4.0/).
Copyright: This open access article is published under a Creative Commons CC BY 4.0 license, which permit the free download, distribution, and reuse, provided that the author and preprint are cited in any reuse.