3. Results and Discussion
3.1. Powder X-Ray Diffraction Characteristics of the Synthesized ZnIM Material
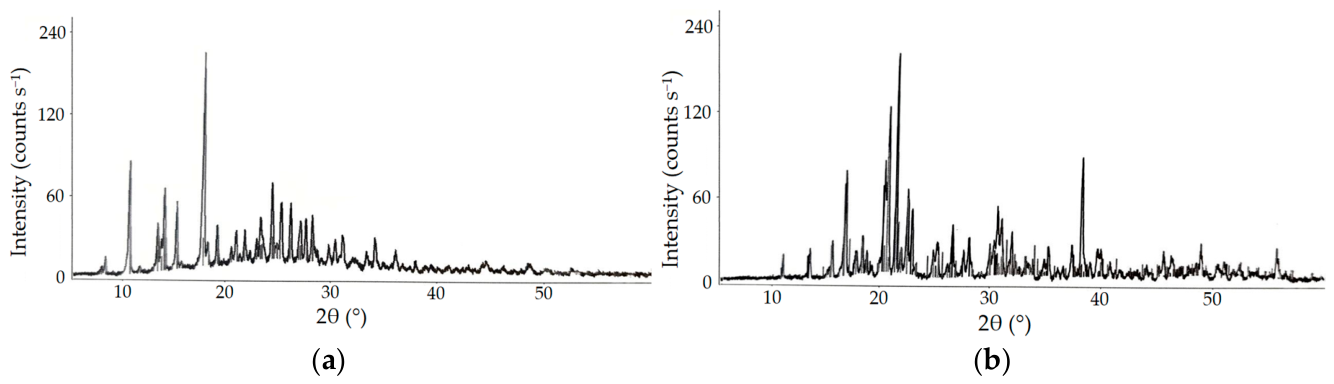
The PXRD patterns of free imatinib and the synthesized ZnIM material differed substantially (
Figure 1). Free imatinib exhibited a well-defined crystalline diffraction profile dominated by a sharp reflection at approximately 18° 2θ, together with prominent reflections around 11°, 14–15°, and within the 23–28° 2θ region. In contrast, the synthesized ZnIM material displayed a markedly different distribution of diffraction intensities, with its most intense reflections occurring at approximately 21–22° 2θ, accompanied by a prominent reflection near 38° 2θ and numerous changes in peak positions and relative intensities throughout the recorded range. The pronounced redistribution of diffraction features indicates that the synthesized material possesses a crystalline organization distinct from that of the starting imatinib and is consistent with the formation of a new solid-state phase following reaction with ZnCl
2.
Imatinib is a conformationally flexible molecule, and its solid-state conformation and crystal packing can vary depending on intra- and intermolecular interactions [
23,
24]. Distinct crystalline forms of imatinib mesylate have likewise been shown to exhibit different molecular conformations and PXRD characteristics [
25]. In addition, complexation of imatinib mesylate with divalent Co(II), Cu(II), and Ni(II) ions has been reported to yield products with physicochemical characteristics distinct from those of the parent compound [
15]. These findings provide a chemical basis for interpreting the marked alteration of the diffraction profile observed after reaction of imatinib with ZnCl
2. However, PXRD alone does not establish the Zn(II) coordination site, molecular geometry, exact stoichiometry, or definitive phase purity of the synthesized material. The present diffraction data should therefore be regarded as supporting the formation of the proposed ZnIM complex rather than providing complete structural confirmation.
3.2. Effect of the Imatinib–Zinc Complex on Seed Germination and Germination Energy
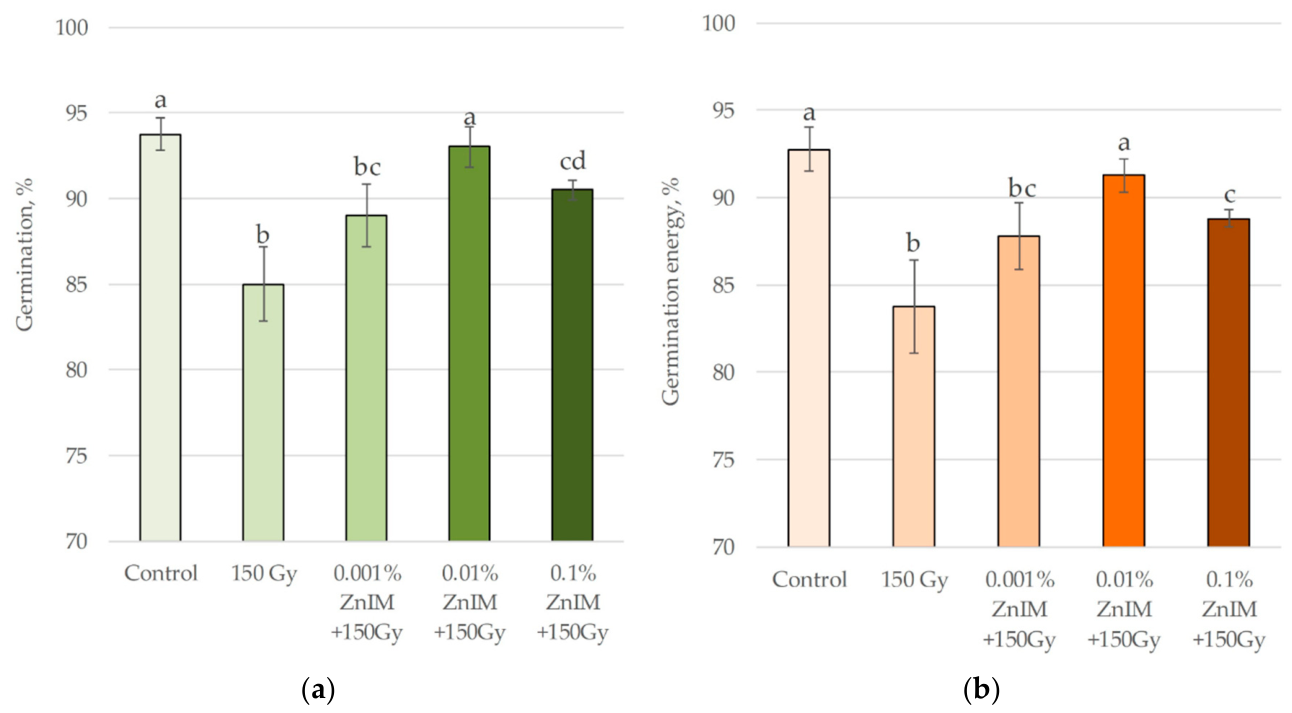
Seed germination and germination energy provide sensitive measures of seed viability and the capacity for rapid establishment under stress. In the present study, exposure of maize seeds to 150 Gy gamma irradiation significantly impaired both parameters (
Figure 2). Final germination decreased from 93.8 ± 1.0% in the non-irradiated control to 85.0 ± 2.2% following irradiation, corresponding to a reduction of 8.8 percentage points, or approximately 9.3% relative to the control. Germination energy showed a comparable response, declining from 92.8 ± 1.3% to 83.8 ± 2.6%, a decrease of 9.0 percentage points, or approximately 9.7%. The statistical separation of the control and 150 Gy treatments confirms that irradiation at this dose significantly reduced both the final proportion of germinated seeds and the proportion capable of germinating rapidly during the early phase of the assay.
The inhibitory effect observed at 150 Gy is consistent with previous studies demonstrating dose-dependent suppression of germination and early development in irradiated maize. Gamma irradiation has been reported to reduce germination percentage and germination index progressively with increasing absorbed dose, together with inhibition of subsequent root and shoot growth [
6]. More recent work involving several maize genotypes similarly demonstrated declining germination with increasing gamma-radiation exposure and estimated a mean lethal dose of 254.3 Gy, while also revealing substantial genotypic differences in radiation sensitivity [
7]. In this context, the approximately 9–10% reduction observed at 150 Gy in the present study is consistent with a substantial but non-lethal stress level that was sufficient to impair the physiological processes governing rapid and successful germination.
Seed pre-treatment with ZnIM partially counteracted the inhibitory effects of gamma irradiation, but the magnitude of recovery differed markedly among concentrations. At the lowest concentration, 0.001% ZnIM increased final germination from 85.0 ± 2.2% to 89.0 ± 0.6% and germination energy from 83.8 ± 2.6% to 87.8 ± 1.9%. Both parameters therefore increased by 4.0 percentage points relative to irradiation alone. However, the 0.001% treatment shared statistical-group letters with the untreated 150 Gy treatment for both variables, indicating that these numerical improvements were not statistically significant at p < 0.05. Thus, the lowest ZnIM concentration produced only a modest tendency toward recovery and was insufficient to provide statistically supported protection of germination performance.
A substantially stronger response was obtained with 0.01% ZnIM. Final germination reached 93.0 ± 1.2%, representing an increase of 8.0 percentage points, or approximately 9.4%, relative to irradiated untreated seeds. Germination energy increased to 91.3 ± 1.0%, corresponding to an improvement of 7.5 percentage points, or approximately 9.0%, compared with the 150 Gy treatment. Importantly, both parameters were statistically indistinguishable from the non-irradiated control. These results indicate that 0.01% ZnIM largely reversed the irradiation-induced decline in germination performance and restored both final germination and early germination capacity to values comparable with those of non-irradiated seeds. Among the concentrations tested, this treatment therefore provided the clearest evidence of protection during the germination phase.
Increasing the ZnIM concentration to 0.1% did not further enhance the response. Final germination reached 90.5 ± 1.8%, whereas germination energy increased to 88.8 ± 0.5%. Relative to irradiation alone, these values represented improvements of approximately 6.5% and 6.0%, respectively. Both parameters were significantly higher than those in the untreated 150 Gy group, demonstrating a statistically detectable protective effect. However, the 0.1% treatment also remained significantly below the non-irradiated control for both germination and germination energy. Thus, although 0.1% ZnIM partially alleviated radiation-induced inhibition, it was less effective than 0.01% ZnIM and did not restore seed performance to the control level.
Taken together, these responses reveal a clear non-linear concentration–response relationship. Increasing ZnIM from 0.001% to 0.01% substantially enhanced protection, whereas a further ten-fold increase to 0.1% reduced rather than strengthened the recovery of both germination variables. The superior performance of the intermediate concentration therefore suggests the existence of an effective physiological range within which ZnIM provides maximal benefit during seed germination. This pattern is particularly relevant for Zn-containing treatments because Zn is essential for plant metabolism but becomes inhibitory when supplied above an appropriate physiological range. Consequently, greater ZnIM exposure cannot be assumed to produce greater protection.
The beneficial response to ZnIM is broadly consistent with previous studies showing that Zn-containing seed treatments can enhance maize establishment under unfavorable conditions. Micronutrient seed priming containing Zn has been reported to accelerate maize emergence and improve subsequent crop establishment and performance [
10]. Similarly, combined priming with Zn and glutathione improved maize germination and seedling vigor under water-deficit conditions, together with changes in reserve metabolism and antioxidant activity [
26]. Although these studies involved stresses and formulations different from those used here, they support the broader concept that pre-sowing exposure to an appropriately selected Zn-containing treatment can increase the capacity of maize seeds to maintain germination processes under adverse conditions.
Because ZnIM was applied before irradiation and germination, a seed-priming-related contribution to the observed response is biologically plausible. During imbibition, successful germination requires rapid membrane reorganization, restoration of mitochondrial activity, mobilization of stored reserves, activation of enzyme systems, and maintenance of cellular redox balance. Partial preservation of these processes could contribute to the higher germination and germination energy observed in ZnIM-treated irradiated seeds. The accompanying reduction in MDA detected later in seedling development in the present study also supports an association between ZnIM treatment and lower oxidative membrane injury. Nevertheless, membrane integrity, ROS concentrations, reserve mobilization, antioxidant enzyme activities, and other processes operating directly during seed imbibition were not measured. These mechanisms should therefore be regarded as biologically plausible explanations rather than experimentally demonstrated pathways.
An additional limitation is that the experimental design did not include non-irradiated seeds treated with ZnIM, free imatinib, a Zn salt alone, or a non-coordinated mixture of imatinib and Zn. Consequently, the present data cannot distinguish whether the improvement in germination resulted specifically from the intact ZnIM complex, from Zn availability, from the imatinib ligand, from a general seed-priming effect, or from interactions among these factors. The results nevertheless demonstrate that pre-treatment with the synthesized ZnIM formulation before irradiation significantly modified the response of maize seeds to 150 Gy gamma radiation.
Overall, gamma irradiation significantly reduced both final germination and germination energy, whereas ZnIM pre-treatment alleviated these effects in a strongly concentration-dependent but non-linear manner. The 0.001% treatment produced only numerical improvement, whereas 0.1% ZnIM provided significant but incomplete protection. In contrast, 0.01% ZnIM restored both germination parameters to values statistically comparable with the non-irradiated control. These findings identify 0.01% ZnIM as the most effective concentration tested for preserving maize seed germination performance following exposure to 150 Gy gamma irradiation.
3.3. Effect of the Imatinib–Zinc Complex on Root and Shoot Growth
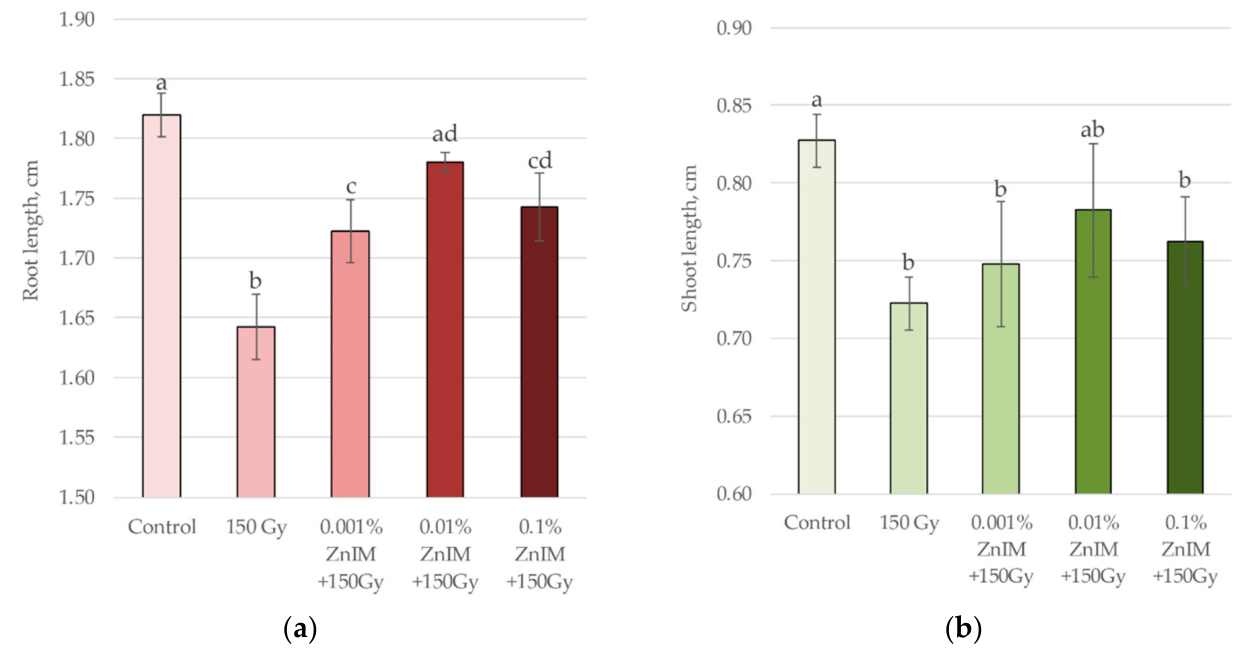
Root and shoot elongation are sensitive indicators of early seedling performance because both processes depend on sustained cell division, cell expansion, reserve mobilization, and maintenance of cellular homeostasis during establishment. In the present study, exposure of maize seeds to 150 Gy gamma irradiation significantly inhibited both root and shoot growth (
Figure 3). Mean root length decreased from 1.82 ± 0.02 cm in the non-irradiated control to 1.643 ± 0.03 cm after irradiation, corresponding to a reduction of approximately 9.8%. Shoot length declined from 0.828 ± 0.02 to 0.723 ± 0.02 cm, representing a reduction of approximately 12.7%. The statistical separation between the control and 150 Gy treatments for both parameters confirms that irradiation substantially impaired early seedling elongation.
The magnitude of growth inhibition observed here is consistent with previous findings in gamma-irradiated maize. Marcu et al. reported that exposure of maize seeds to 100 Gy reduced root and shoot lengths by approximately 9% and 11%, respectively, with progressively stronger inhibition at higher radiation doses [
6]. The similarity between those responses and the reductions recorded in the present experiment further supports the sensitivity of early maize seedling growth to moderate gamma-radiation exposure. The somewhat greater proportional reduction in shoot length than in root length observed here also indicates that individual seedling organs may differ in their sensitivity to irradiation.
ZnIM pre-treatment produced a clear protective response in root development. The lowest concentration, 0.001% ZnIM, increased root length to 1.723 ± 0.03 cm, approximately 4.9% above that of irradiated untreated seedlings. Treatment with 0.1% ZnIM increased root length to 1.743 ± 0.03 cm, representing an improvement of approximately 6.1% relative to irradiation alone. Both treatments differed significantly from the 150 Gy group, demonstrating that even the lowest tested ZnIM concentration provided statistically detectable protection of root elongation. Nevertheless, root lengths following 0.001% and 0.1% ZnIM remained significantly below the non-irradiated control, indicating incomplete recovery.
The strongest response was observed with 0.01% ZnIM. Root length increased to 1.78 ± 0.01 cm, approximately 8.4% above the value recorded after irradiation alone and only about 2.2% below the non-irradiated control. According to the statistical grouping in
Figure 3a, this treatment differed significantly from the untreated 150 Gy group but not from the control. Thus, 0.01% ZnIM restored root elongation to a level statistically comparable with that of non-irradiated seedlings. This finding closely parallels the germination response described above, in which the same concentration provided the greatest recovery of both final germination and germination energy.
Shoot growth exhibited a similar numerical concentration pattern but a weaker statistical response. Shoot length increased from 0.723 ± 0.02 cm in irradiated untreated seedlings to 0.748 ± 0.04 cm after treatment with 0.001% ZnIM, corresponding to an increase of approximately 3.5%. Treatment with 0.01% ZnIM increased shoot length to 0.783 ± 0.04 cm, approximately 8.3% above the irradiated value, whereas 0.1% ZnIM resulted in a shoot length of 0.763 ± 0.03 cm, an increase of approximately 5.5%.
Despite these numerical improvements, none of the ZnIM treatments differed significantly from the irradiated untreated group in shoot length. The 0.001% and 0.1% treatments remained in the same statistical group as the 150 Gy treatment, whereas 0.01% ZnIM occupied an intermediate statistical position and did not differ significantly from either the irradiated group or the non-irradiated control. Consequently, the shoot data indicate a tendency toward partial recovery, particularly at 0.01% ZnIM, but do not provide statistically conclusive evidence that ZnIM restored shoot elongation under the conditions tested.
The contrasting root and shoot responses are an important feature of the present results. Whereas all three ZnIM concentrations significantly improved root length relative to irradiation alone, the corresponding improvements in shoot length remained statistically unresolved. This suggests that early root development was more responsive to ZnIM pre-treatment than shoot development. Such an organ-specific response is biologically plausible because roots are the first actively elongating organs to emerge during germination and are directly dependent on the physiological status established during seed imbibition and early reserve mobilization. A pre-sowing treatment may therefore influence root meristem activity and elongation more rapidly than subsequent shoot development.
The preferential improvement in root growth is broadly consistent with previous studies of Zn-containing seed treatments in maize. Micronutrient seed priming containing Zn has been shown to improve early maize establishment and increase root and shoot biomass under micronutrient-deficient conditions [
11]. Likewise, seed-applied Zn/Mn treatments promoted root development and partially alleviated growth inhibition in maize subjected to low-temperature stress; these effects were accompanied by improved micronutrient status and enhanced antioxidant enzyme activity [
27]. Although these studies involved different stressors and Zn formulations, they support the broader concept that appropriately applied Zn-containing seed treatments can preferentially benefit early root establishment under adverse conditions.
Several physiological processes could contribute to the observed preservation of root elongation. Gamma irradiation can interfere with meristematic activity, cellular expansion, membrane integrity, hormonal regulation, and redox homeostasis, all of which are essential for sustained root growth. Altered elongation and changes in indole-3-acetic acid levels have previously been reported in irradiated maize coleoptiles [
28]. In the present study, ZnIM may have helped preserve processes required for root meristem function by limiting oxidative injury or improving Zn availability during early development. However, cell-division rates, meristem structure, hormone concentrations, Zn uptake, ROS levels, and antioxidant enzyme activities were not measured. These explanations should therefore be regarded as mechanistically plausible rather than experimentally demonstrated.
The concentration pattern further reinforces the non-linear response observed for germination. Increasing ZnIM concentration from 0.001% to 0.01% enhanced root recovery, whereas a further increase to 0.1% provided no additional benefit. The same intermediate concentration also produced the largest numerical improvement in shoot length. Thus, the seedling-growth response does not support a simple dose-dependent relationship in which greater ZnIM exposure results in progressively greater protection. Instead, 0.01% appears to fall within a more favorable physiological range for preserving early maize growth after irradiation.
Overall, ZnIM pre-treatment provided substantially stronger protection of root growth than of shoot growth following exposure to 150 Gy gamma irradiation. All tested ZnIM concentrations significantly increased root length relative to irradiation alone, with 0.01% ZnIM producing the greatest recovery and restoring root elongation to a value statistically comparable with the non-irradiated control. Shoot length followed the same numerical ranking, with the largest increase at 0.01%, but the treatment effects were not statistically significant relative to irradiation alone. Together with the germination results, these findings identify 0.01% ZnIM as the most consistently effective concentration for preserving early maize establishment under the applied radiation stress.
3.5. Effects of the Imatinib–Zinc Complex on Photosynthetic Pigments and PSII Efficiency
Photosynthetic pigment content and chlorophyll fluorescence provide complementary information on the structural and functional status of the photosynthetic apparatus under stress. In the present study, exposure of maize seeds to 150 Gy gamma irradiation markedly altered both pigment accumulation and the maximum quantum efficiency of photosystem II (PSII) in the resulting seedlings (
Table 1;
Figure 5). Irradiation significantly reduced chlorophyll
a, chlorophyll
b, total chlorophyll, and carotenoid contents and was accompanied by a significant decrease in Fv/Fm. Together, these responses indicate that the applied radiation dose affected both the accumulation of light-harvesting pigments and the photochemical efficiency of PSII.
Chlorophyll
a showed the strongest pigment response to irradiation. Its content decreased from 2.75 ± 0.04 mg g
−1 fresh weight in the non-irradiated control to 1.87 ± 0.04 mg g
−1 following exposure to 150 Gy, corresponding to a reduction of approximately 32.0%. This pronounced decline is consistent with previous observations in gamma-irradiated maize, in which increasing radiation doses progressively reduced chlorophyll
a, chlorophyll
b, and carotenoid contents [
6]. The present results therefore confirm that chlorophyll accumulation is highly sensitive to radiation stress during early maize development.
The response of chlorophyll a to ZnIM depended strongly on treatment concentration. The lowest concentration, 0.001% ZnIM, produced essentially no recovery, with chlorophyll a reaching 1.88 ± 0.04 mg g−1, only approximately 0.5% above the irradiated untreated value. The 0.001% treatment remained in the same statistical group as the 150 Gy treatment, indicating that this concentration did not significantly preserve chlorophyll a accumulation.
In contrast, 0.01% and 0.1% ZnIM produced significant recovery. Treatment with 0.01% ZnIM increased chlorophyll a content to 2.28 ± 0.05 mg g−1, approximately 21.9% above the value recorded after irradiation alone. The 0.1% treatment increased chlorophyll a to 2.16 ± 0.07 mg g−1, representing an improvement of approximately 15.5%. Both treatments differed significantly from the untreated 150 Gy group, although neither restored chlorophyll a to the non-irradiated control level. The largest recovery was therefore obtained with 0.01% ZnIM, again indicating that the intermediate concentration was more effective than the highest concentration tested.
Chlorophyll b exhibited a different response. Irradiation reduced chlorophyll b content from 0.900 ± 0.055 to 0.673 ± 0.051 mg g−1, corresponding to a decrease of approximately 25.2%. ZnIM treatment increased chlorophyll b numerically to 0.680 ± 0.037, 0.750 ± 0.044, and 0.730 ± 0.037 mg g−1 at 0.001%, 0.01%, and 0.1%, respectively. These values represented increases of approximately 1.0%, 11.4%, and 8.5% relative to irradiation alone. However, all irradiated treatments shared the same statistical grouping for chlorophyll b. Thus, despite the numerical improvement observed particularly at 0.01% ZnIM, the data do not provide statistically significant evidence that ZnIM restored chlorophyll b accumulation.
The contrasting responses of chlorophyll a and chlorophyll b suggest that ZnIM did not affect all pigment components uniformly. Chlorophyll a is the principal pigment associated with the PSII and PSI reaction centers and core antenna complexes, whereas chlorophyll b is predominantly associated with peripheral light-harvesting complexes. The stronger recovery of chlorophyll a may therefore reflect differential preservation or recovery of components within the photosynthetic apparatus. However, the abundance and organization of individual pigment–protein complexes were not measured, and this interpretation should therefore be regarded as a hypothesis rather than a demonstrated mechanism.
Total chlorophyll content closely reflected the response of chlorophyll a. Gamma irradiation reduced total chlorophyll from 3.65 ± 0.09 to 2.54 ± 0.04 mg g−1, a decrease of approximately 30.4%. Treatment with 0.001% ZnIM produced little change, resulting in 2.56 ± 0.08 mg g−1 and no significant difference from irradiation alone. The strongest recovery was again observed with 0.01% ZnIM, which increased total chlorophyll to 3.03 ± 0.03 mg g−1, approximately 19.3% above the 150 Gy value and significantly higher than the irradiated untreated treatment. Treatment with 0.1% ZnIM increased total chlorophyll numerically to 2.89 ± 0.10 mg g−1, an improvement of approximately 13.8%; however, this treatment shared statistical-group letters with both the 150 Gy and 0.01% ZnIM groups, indicating an intermediate response that was not clearly separable from irradiation alone.
The greater effectiveness of the intermediate ZnIM concentration is biologically consistent with the importance of Zn in chloroplast development and pigment metabolism. Transcriptomic and proteomic studies in maize have shown that Zn deficiency disrupts genes and proteins involved in chlorophyll biosynthesis, thylakoid organization, chloroplast structure, and photosynthetic electron transport [
9,
32]. These studies support the broader concept that adequate Zn availability is important for maintaining the structural and functional integrity of the photosynthetic apparatus. Nevertheless, because the present experiment did not include Zn-only or imatinib-only treatments, the observed effects cannot be attributed specifically to Zn or distinguished from those of the complete ZnIM formulation.
Carotenoid content was less strongly affected by irradiation than chlorophyll content. Exposure to 150 Gy reduced carotenoids from 0.650 ± 0.029 to 0.580 ± 0.029 mg g−1, corresponding to a decrease of approximately 10.8%. Treatment with 0.001%, 0.01%, and 0.1% ZnIM increased carotenoid content to 0.610 ± 0.029, 0.650 ± 0.037, and 0.630 ± 0.037 mg g−1, respectively. These values represented numerical increases of approximately 5.2%, 12.1%, and 8.6% relative to irradiation alone. Notably, the mean carotenoid content after 0.01% ZnIM was equal to that of the non-irradiated control. However, all ZnIM-treated groups shared statistical letters with the irradiated treatment, indicating that none of these increases was statistically significant. The carotenoid data therefore indicate a tendency toward recovery, but not a statistically confirmed protective effect.
The weaker statistical response of carotenoids compared with chlorophyll a may reflect differences in their sensitivity, turnover, and physiological roles under radiation stress. Carotenoids contribute not only to light harvesting but also to stabilization of pigment–protein complexes and dissipation of excess excitation energy. Their comparatively smaller decline following irradiation may indicate that the total carotenoid pool was less sensitive than chlorophyll accumulation under the present conditions. However, individual carotenoid species, xanthophyll-cycle activity, and antioxidant functions were not measured, so the physiological significance of this apparent stability cannot be resolved from total carotenoid content alone.
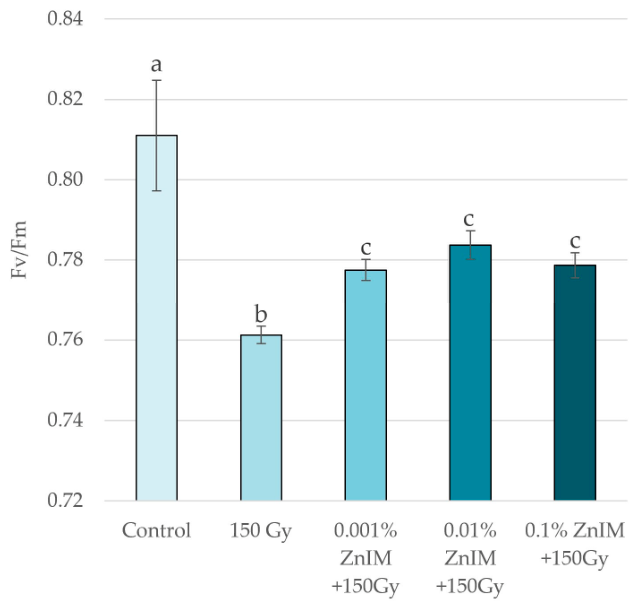
Changes in pigment accumulation were accompanied by a significant reduction in PSII photochemical efficiency. Fv/Fm decreased from 0.811 ± 0.014 in the non-irradiated control to 0.761 ± 0.002 following 150 Gy irradiation, corresponding to a reduction of approximately 6.2% (
Figure 5). The significant statistical separation between these treatments demonstrates that gamma irradiation impaired the maximum quantum efficiency of PSII.
The proportional decrease in Fv/Fm was substantially smaller than the decrease in chlorophyll a or total chlorophyll. This difference indicates that pigment accumulation and PSII photochemical efficiency responded to radiation stress with different magnitudes. A reduction in total pigment abundance does not necessarily produce an equivalent decline in Fv/Fm because this fluorescence parameter reflects the maximum photochemical efficiency of functional PSII reaction centers after dark adaptation rather than the total quantity of photosynthetic pigments present in the leaf.
All three ZnIM concentrations significantly improved Fv/Fm relative to irradiation alone. Treatment with 0.001% ZnIM increased Fv/Fm to 0.778 ± 0.003, approximately 2.2% above the irradiated value. The 0.01% and 0.1% treatments increased Fv/Fm to 0.784 ± 0.004 and 0.779 ± 0.003, corresponding to improvements of approximately 3.0% and 2.4%, respectively. All ZnIM-treated groups differed significantly from the 150 Gy treatment, whereas no significant differences were detected among the three ZnIM concentrations. Thus, in contrast to pigment accumulation, for which statistically significant recovery was concentrated mainly at 0.01% and 0.1% ZnIM, PSII efficiency responded positively even to the lowest concentration tested.
Despite this improvement, none of the ZnIM treatments restored Fv/Fm completely to the non-irradiated control. Relative to the control value, Fv/Fm remained approximately 4.1%, 3.3%, and 3.9% lower following 0.001%, 0.01%, and 0.1% ZnIM treatment, respectively. The statistical grouping likewise separated all ZnIM-treated groups from the control. ZnIM therefore provided partial but not complete preservation of PSII photochemical efficiency.
The highest numerical Fv/Fm value was obtained with 0.01% ZnIM, which also produced the highest chlorophyll a, chlorophyll b, total chlorophyll, and carotenoid values among irradiated treatments. This convergence across pigment and fluorescence measurements identifies 0.01% ZnIM as the concentration associated with the broadest preservation of photosynthetic performance. Particularly noteworthy is the response to 0.001% ZnIM: this treatment significantly improved Fv/Fm despite producing no significant recovery of chlorophyll a, chlorophyll b, or total chlorophyll. This dissociation suggests that preservation of PSII photochemical efficiency can occur even when pigment accumulation remains strongly constrained, although the mechanism underlying this response cannot be determined from Fv/Fm alone.
Protective effects of Zn-containing formulations on photosynthesis have also been reported under other types of plant stress. Foliar application of ZnO nanoparticles improved photosynthetic performance and PSII photochemical efficiency in salt-stressed maize, with effectiveness varying according to treatment concentration [
33]. A Zn-containing polyphenolic complex has likewise been reported to preserve Fv/Fm and photosynthetic pigment pools in maize challenged with
Bipolaris maydis [
34]. Although these studies involved stressors and formulations different from those used in the present experiment, they support the broader concept that appropriately selected Zn-containing treatments can contribute to maintenance of photosynthetic function under adverse conditions.
The overall concentration response was again non-linear. Increasing ZnIM from 0.001% to 0.01% enhanced chlorophyll recovery and produced the highest numerical Fv/Fm value, whereas increasing the concentration further to 0.1% provided no additional benefit. The 0.01% treatment consistently produced the highest mean values for all measured pigment variables and Fv/Fm among irradiated plants. This pattern agrees with the germination and root-growth results and reinforces the interpretation that the intermediate ZnIM concentration was within a more favorable physiological range than the highest concentration tested. The importance of Zn concentration is well established, because adequate Zn supports chloroplast structure and photosynthetic metabolism, whereas excessive Zn exposure can disrupt pigment metabolism and other physiological processes [
35,
36].
The mechanisms underlying the observed preservation of photosynthetic traits cannot be established from the present measurements alone. Reduced lipid peroxidation, stabilization of chloroplast membranes, improved Zn availability, maintenance of pigment biosynthesis, or enhanced protection and repair of PSII components could all contribute to the observed response. The concomitant reduction in MDA, particularly at 0.01% and 0.1% ZnIM, is consistent with an association between lower oxidative membrane injury and better preservation of photosynthetic function. However, chloroplast ultrastructure, pigment-biosynthesis enzymes, electron transport rates, non-photochemical quenching, gas exchange, ROS concentrations, antioxidant enzyme activities, and PSII protein abundance were not measured. These possible mechanisms should therefore be considered testable interpretations rather than experimentally established pathways.
Overall, 150 Gy gamma irradiation caused a pronounced reduction in photosynthetic pigment accumulation and a smaller but statistically significant decline in the maximum quantum efficiency of PSII. ZnIM partially mitigated both effects, although the response differed among photosynthetic parameters. Chlorophyll a and total chlorophyll showed the clearest pigment recovery, whereas chlorophyll b and carotenoid increases were numerical but not statistically significant. In contrast, all three ZnIM concentrations significantly improved Fv/Fm, although full recovery to the control level was not achieved. Among the concentrations tested, 0.01% ZnIM provided the most consistent overall preservation of the photosynthetic apparatus, producing the highest pigment contents and the highest numerical Fv/Fm among irradiated seedlings.
3.6. Effects of the Imatinib–Zinc Complex on Morphological and Yield-Related Traits
Morphological and yield-related traits provide an integrated assessment of whether physiological protection observed during germination and early seedling development persists through later stages of plant growth. In the present study, the long-term response to 150 Gy gamma irradiation differed markedly among the four measured traits (
Table 2). Leaf area and cob length remained statistically unchanged, whereas plant height and 1000-grain weight were significantly reduced. This differential response indicates that the applied radiation dose did not uniformly affect all components of maize development but exerted a clearer influence on vegetative stature and grain filling.
Leaf area showed only minor numerical variation among treatments. The mean value decreased from 54.6 ± 0.3 cm2 in the non-irradiated control to 53.8 ± 0.5 cm2 after exposure to 150 Gy, corresponding to a reduction of approximately 1.5%. Pre-treatment with 0.001%, 0.01%, and 0.1% ZnIM resulted in leaf areas of 53.7 ± 0.4, 53.9 ± 0.2, and 53.9 ± 0.3 cm2, respectively. All treatments shared the same statistical grouping, demonstrating that neither irradiation nor ZnIM pre-treatment significantly affected leaf area under the conditions of the experiment. Thus, despite the significant effects of irradiation on several early physiological parameters, final leaf expansion remained comparatively stable.
Cob length exhibited a similarly limited response. Exposure to 150 Gy reduced mean cob length from 19.9 ± 0.3 cm in the control to 19.4 ± 0.3 cm, a numerical decrease of approximately 2.5%. Values of 19.3 ± 0.3, 19.3 ± 0.2, and 19.5 ± 0.2 cm were recorded following treatment with 0.001%, 0.01%, and 0.1% ZnIM, respectively. Because all groups belonged to the same statistical category, none of these differences was significant. These results indicate that longitudinal cob development was relatively insensitive to both 150 Gy irradiation and ZnIM treatment in the maize genotype examined.
In contrast to leaf area and cob length, 1000-grain weight was significantly affected by irradiation. The value decreased from 315 ± 5 g in the non-irradiated control to 298 ± 5 g after exposure to 150 Gy, corresponding to a reduction of approximately 5.4%. The statistical separation of these treatments indicates that irradiation had a persistent negative effect on grain filling or final kernel mass, even though cob length itself remained unchanged. This distinction suggests that reproductive structures could attain a similar external size while accumulating less grain mass.
The lowest ZnIM concentration did not alleviate this effect. Treatment with 0.001% ZnIM resulted in a 1000-grain weight of 297 ± 3 g, essentially identical to that of irradiated untreated plants and significantly lower than the control. In contrast, 0.01% ZnIM increased 1000-grain weight to 304 ± 3 g, while 0.1% ZnIM increased it to 307 ± 3 g. Relative to the 150 Gy treatment, these values represented numerical improvements of approximately 2.0% and 3.0%, respectively.
The statistical designation ab assigned to the 0.01% and 0.1% treatments is particularly important for interpretation. Both treatments were statistically indistinguishable from the non-irradiated control, but they were also statistically indistinguishable from the irradiated untreated group. Consequently, these intermediate values cannot be described as statistically significant recovery relative to irradiation alone. Instead, they indicate a numerical tendency toward partial restoration of grain mass. Among the irradiated treatments, 0.1% ZnIM produced the highest mean 1000-grain weight, although it was not statistically superior to 0.01% ZnIM.
Plant height showed the strongest long-term response to irradiation among the morphological traits examined. Mean plant height decreased from 198 ± 4 cm in the non-irradiated control to 176 ± 2 cm following exposure to 150 Gy. This represented a reduction of 22 cm, or approximately 11.1%, and the difference was statistically significant. The persistence of this effect to maturity indicates that the consequences of seed irradiation extended well beyond germination and early seedling development and influenced subsequent vegetative growth.
The 0.001% ZnIM treatment provided essentially no recovery of plant height. Plants in this group reached 177 ± 3 cm, only approximately 0.6% taller than irradiated untreated plants, and both treatments shared the same statistical grouping. In contrast, plants receiving 0.01% ZnIM reached 188 ± 5 cm, representing an increase of approximately 6.8% relative to the 150 Gy treatment. Treatment with 0.1% ZnIM resulted in a mean height of 186 ± 3 cm, approximately 5.7% above that of untreated irradiated plants.
As observed for 1000-grain weight, the 0.01% and 0.1% treatments were assigned the intermediate statistical designation ab. Their mean plant heights therefore did not differ significantly from either the non-irradiated control or the untreated 150 Gy treatment. These values should consequently be interpreted as trends toward partial recovery rather than statistically confirmed protection of final plant height. Numerically, 0.01% ZnIM produced the greatest recovery, restoring approximately 55% of the height difference between the irradiated and non-irradiated treatments.
The reduction in plant height and 1000-grain weight is consistent with the well-established dose dependence of gamma-radiation effects in maize. Recent field experiments have shown that relatively low radiation doses may stimulate certain growth and yield-related traits, whereas exposures of 100 Gy and above can progressively reduce plant height, cob characteristics, grain mass, and yield [
37]. Earlier studies likewise demonstrated dose-dependent changes in maize survival, plant height, and grain production following gamma irradiation [
38]. The reductions observed at 150 Gy in the present experiment are therefore consistent with exposure above the range in which hormetic stimulation would be expected to dominate.
Several processes could contribute to the persistent reduction in plant height and grain mass. Ionizing radiation can interfere with cell proliferation and expansion, assimilate production, nutrient transport, reproductive development, and allocation of photoassimilates to developing kernels. At sufficiently high doses, radiation-induced oxidative and cytogenetic damage may further constrain plant growth and reproductive performance. In maize, radiation doses above the stimulatory range have been associated with reductions in growth and yield-related traits as well as increased cytogenetic abnormalities [
6,
37]. However, cell division, chromosome damage, assimilate partitioning, and reproductive physiology were not measured in the present study, and these processes should therefore be regarded as plausible explanations rather than experimentally demonstrated mechanisms.
The numerical recovery observed with 0.01% and 0.1% ZnIM is also biologically compatible with the established importance of Zn in maize growth and reproductive development. Zinc fertilization can increase maize grain yield and kernel weight, although the magnitude of the response depends strongly on application rate, timing, genotype, soil Zn status, and environmental conditions [
39,
40,
41]. Zn supply may also influence dry-matter accumulation and translocation from vegetative tissues to developing kernels, processes that are important for final grain filling [
40].
Nevertheless, the response observed here was substantially weaker than the significant improvements commonly reported following conventional Zn fertilization. This difference is not unexpected because ZnIM was applied only once as a pre-irradiation seed treatment rather than supplied continuously through the soil or foliage during plant development. The treatment may therefore have exerted its strongest influence during seed imbibition, germination, and early seedling establishment, with progressively weaker residual effects as plants approached maturity. Differences in Zn formulation, application method, genotype, soil conditions, and stress type further limit direct comparison with conventional Zn-fertilization studies.
This interpretation is consistent with the broader response pattern observed throughout the present experiment. ZnIM produced statistically supported effects on several early and intermediate traits, including germination, germination energy, root elongation, MDA accumulation, chlorophyll a, total chlorophyll, and Fv/Fm. By contrast, its effects on mature-plant height and 1000-grain weight were numerical rather than statistically significant relative to irradiation alone. Thus, the early physiological and biochemical protection associated with ZnIM did not translate proportionally into statistically confirmed improvement of all mature-plant traits.
The concentration response at maturity also differed somewhat from that observed during early development. The 0.01% treatment produced the greatest numerical recovery of plant height, whereas 0.1% ZnIM produced the highest mean 1000-grain weight. The 0.001% treatment provided essentially no improvement in either trait. These data suggest that concentrations of 0.01% and 0.1% were more biologically responsive than 0.001% for the mature traits examined; however, because neither concentration differed significantly from the irradiated untreated treatment, the present results do not establish a statistically optimal ZnIM concentration for mature-plant performance.
The interpretation of these mature-plant responses should also account for experimental power and the scope of the measured yield variables. The field experiment included four biological replicates, and the intermediate statistical groupings observed for plant height and 1000-grain weight indicate that treatment means were not sufficiently separated to demonstrate significant recovery. Moreover, 1000-grain weight represents only one component of crop productivity. Grain yield per plant or per unit area, kernel number per cob, harvest index, and total biomass were not determined. Consequently, the present data cannot establish whether ZnIM improved overall maize yield under radiation stress. Larger field experiments incorporating these additional agronomic endpoints would be required to determine whether the numerical improvements observed at 0.01% and 0.1% ZnIM are reproducible and agronomically meaningful.
Overall, exposure to 150 Gy gamma irradiation significantly reduced plant height and 1000-grain weight but did not significantly affect leaf area or cob length. The lowest ZnIM concentration, 0.001%, provided no detectable long-term protection. Treatments with 0.01% and 0.1% ZnIM produced intermediate numerical recovery of plant height and grain mass, but these improvements were not statistically significant relative to irradiation alone. The mature-plant data therefore support a tendency toward partial preservation of vegetative growth and grain filling rather than definitive evidence that ZnIM enhanced final maize productivity under radiation stress. Together with the stronger responses observed during germination and early seedling development, these findings suggest that the principal protective effects of ZnIM were expressed during the earlier stages of plant establishment.
3.4. Temporal Dynamics of Malondialdehyde Accumulation
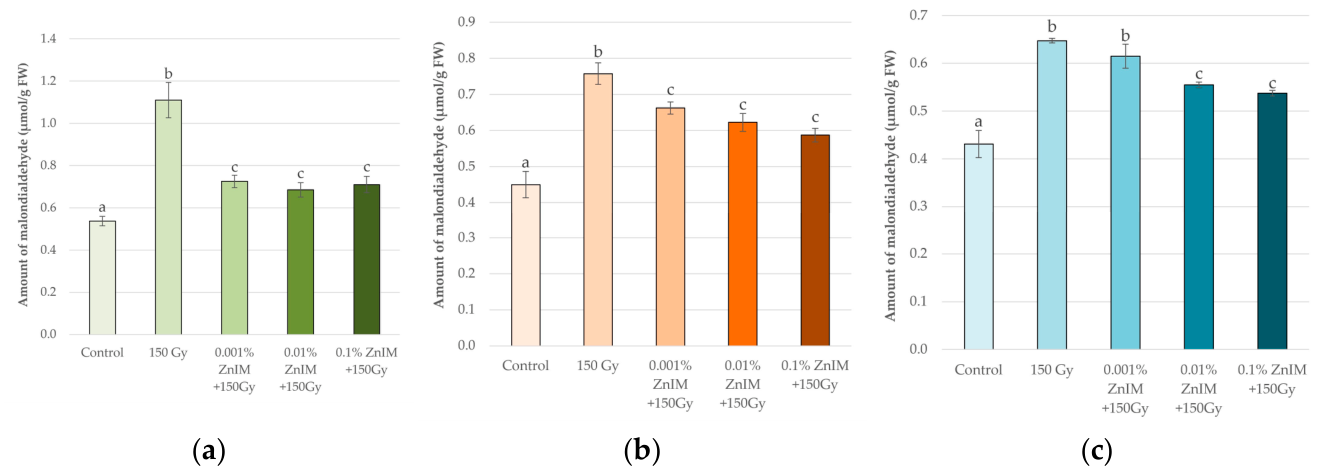
Malondialdehyde (MDA), a product of membrane lipid peroxidation, is widely used as an indicator of oxidative membrane injury in plants. In the present study, exposure of maize seeds to 150 Gy gamma irradiation resulted in significantly elevated MDA content at each of the three sampling periods, demonstrating that radiation-induced oxidative injury persisted during early seedling development (
Figure 4). This response is consistent with the established role of ionizing radiation in promoting reactive oxygen species (ROS) formation and subsequent oxidation of membrane lipids and other cellular components [
1]. Increased MDA accumulation has likewise been reported in gamma-irradiated barley seedlings, with the magnitude of the response varying according to radiation dose and genotype [
29].
The strongest irradiation-associated increase in MDA was observed descriptively during the first week. MDA content increased from 0.538 ± 0.022 nmol g−1 fresh weight in the non-irradiated control to 1.110 ± 0.083 nmol g−1 after exposure to 150 Gy. This represented an increase of approximately 106.3%, or a 2.06-fold elevation relative to the control. The clear statistical separation between the control and irradiated treatments indicates substantial membrane lipid peroxidation during the earliest stage examined. The magnitude of this response further suggests that the initial phase of seedling development was particularly vulnerable to the oxidative consequences of seed irradiation.
ZnIM pre-treatment markedly reduced MDA accumulation during the first week. MDA content decreased to 0.725 ± 0.039 nmol g−1 following treatment with 0.001% ZnIM, 0.685 ± 0.034 nmol g−1 with 0.01% ZnIM, and 0.710 ± 0.030 nmol g−1 with 0.1% ZnIM. Relative to irradiated untreated seedlings, these values represented reductions of approximately 34.7%, 38.3%, and 36.0%, respectively. All three ZnIM treatments had significantly lower MDA levels than the 150 Gy treatment, demonstrating that even the lowest concentration significantly limited irradiation-associated lipid peroxidation during the first week. Nevertheless, MDA remained significantly above the non-irradiated control in all ZnIM-treated groups, indicating partial rather than complete protection. Among the tested concentrations, 0.01% ZnIM produced the lowest numerical MDA value during this initial period.
Radiation-associated lipid peroxidation remained evident during the second week. MDA content in irradiated untreated seedlings was 0.758 ± 0.030 nmol g−1, compared with 0.450 ± 0.037 nmol g−1 in the non-irradiated control, corresponding to an increase of approximately 68.4%. Although the magnitude of the difference was descriptively smaller than that observed during the first week, irradiated seedlings still contained significantly more MDA than control plants. Thus, the biochemical consequences of seed irradiation were not restricted to the immediate post-germination period but remained detectable during subsequent seedling development.
All three ZnIM concentrations significantly reduced MDA content during the second week, although the relative effectiveness of the treatments differed from that observed during week 1. Treatment with 0.001% ZnIM reduced MDA to 0.663 ± 0.019 nmol g−1, representing a decrease of approximately 12.5% relative to irradiation alone. The 0.01% treatment reduced MDA to 0.623 ± 0.025 nmol g−1, corresponding to a decrease of approximately 17.8%, whereas 0.1% ZnIM produced the lowest value, 0.588 ± 0.017 nmol g−1, representing a reduction of approximately 22.4%. Thus, unlike the first week, when the lowest numerical MDA level occurred at 0.01% ZnIM, the highest concentration produced the greatest numerical reduction during the second week.
A similar pattern persisted during the third week. Irradiated untreated seedlings contained 0.648 ± 0.005 nmol g−1 MDA compared with 0.431 ± 0.028 nmol g−1 in the control, representing an increase of approximately 50.3%. The significant difference between these groups demonstrates that irradiation-associated membrane lipid peroxidation remained detectable three weeks after the seeds had been exposed to gamma radiation.
The effectiveness of ZnIM during the third week showed a clearer concentration-related gradient. Treatment with 0.001% ZnIM resulted in an MDA content of 0.615 ± 0.006 nmol g−1, only approximately 5.1% below the irradiated untreated value, and this treatment did not differ significantly from the 150 Gy group. In contrast, 0.01% and 0.1% ZnIM reduced MDA content to 0.555 ± 0.006 and 0.538 ± 0.025 nmol g−1, respectively, corresponding to reductions of approximately 14.4% and 17.0% relative to irradiation alone. Both treatments maintained statistically significant reductions compared with the untreated irradiated group. The lowest ZnIM concentration therefore failed to provide sustained protection through the third week, whereas the effects of 0.01% and 0.1% remained statistically detectable.
A descriptive comparison across the three sampling periods indicates that absolute MDA content declined progressively in all irradiated treatments. In untreated irradiated seedlings, for example, MDA decreased from 1.110 nmol g−1 in the first week to 0.648 nmol g−1 in the third week, representing an overall descriptive reduction of approximately 41.6%. This pattern could reflect progressive physiological acclimation, activation of endogenous protective systems, developmental changes in tissue composition, or replacement of more severely damaged tissues as seedlings grew. However, the statistical analysis was performed independently within each sampling week. Consequently, differences among weeks were not formally tested and should be interpreted as descriptive temporal trends rather than statistically demonstrated changes over time.
The reduction in MDA following ZnIM treatment is consistent with previous evidence that appropriately selected Zn-containing treatments can attenuate oxidative membrane damage in maize. Biogenic ZnO nanoparticles have been reported to reduce MDA accumulation while improving physiological and biochemical performance in maize seedlings, with treatment effectiveness depending strongly on concentration [
30]. Similarly, nano-ZnO application reduced drought-associated oxidative damage in maize and was accompanied by changes in antioxidant and stress-response metabolism [
31]. Although these studies involved ZnO-based materials and stress conditions different from those used here, they support the broader concept that physiologically appropriate Zn-containing treatments can influence oxidative stress responses in maize. They do not, however, establish that ZnIM and ZnO formulations act through the same biochemical mechanisms.
An important feature of the present results is that the concentration associated with the greatest numerical reduction in MDA changed with seedling development. The 0.01% ZnIM treatment produced the lowest MDA value during the first week, whereas 0.1% ZnIM produced the lowest values during both the second and third weeks. This contrasts with the germination and seedling-growth responses, for which 0.01% ZnIM consistently provided the broadest protection. The MDA data therefore suggest that the concentration–response relationship was not only non-linear but also temporally dynamic. The intermediate concentration appeared particularly effective during the initial oxidative response, whereas the higher concentration was associated with a more sustained reduction in lipid peroxidation at later sampling times.
Several mechanisms could potentially contribute to this temporal pattern. An initially effective concentration may support membrane stabilization, Zn-dependent metabolic processes, or antioxidant readiness during early development, whereas a higher treatment concentration might provide a more persistent Zn-associated effect as seedlings develop. However, the present experiment did not determine Zn uptake, tissue Zn concentration, ZnIM stability or dissociation, ROS concentrations, antioxidant enzyme activities, glutathione or ascorbate status, or membrane permeability. It therefore cannot establish whether the observed decline in MDA resulted from enhanced antioxidant capacity, reduced ROS formation, improved membrane stability, altered Zn availability, a seed-priming effect, or another process. These possibilities should be regarded as hypotheses for subsequent mechanistic investigation.
The MDA results also provide an important biochemical complement to the germination and seedling-growth data. Treatments that reduced irradiation-associated MDA accumulation were generally associated with better early plant performance, particularly at 0.01% ZnIM, which showed the strongest overall recovery of germination, germination energy, and root elongation. This correspondence is consistent with the interpretation that reduced oxidative membrane injury contributed to improved seedling establishment. Nevertheless, because these variables were not subjected to a formal correlation or causal analysis, the relationship should not be interpreted as direct evidence that lower MDA caused the observed growth recovery.
Overall, exposure to 150 Gy gamma irradiation resulted in significantly elevated MDA content during each of the three sampling weeks, providing clear biochemical evidence of persistent irradiation-associated lipid peroxidation in developing maize seedlings. ZnIM pre-treatment significantly reduced MDA accumulation at all concentrations during the first and second weeks, whereas only the 0.01% and 0.1% treatments maintained statistically detectable protection during the third week. The 0.01% treatment produced the strongest numerical response during the initial period, while 0.1% ZnIM showed the most persistent reduction at later sampling times. Thus, reduction of MDA accumulation represents one of the clearest biochemical responses associated with ZnIM treatment and supports the conclusion that the formulation partially mitigated oxidative membrane injury following gamma irradiation.
3.7. Integrated Interpretation, Putative Mechanisms, and Study Limitations
The combined results demonstrate that pre-treatment with the imatinib–zinc complex partially mitigated several adverse effects of 150 Gy gamma irradiation in maize, although the magnitude of protection depended on both ZnIM concentration and the response variable examined. Radiation exposure significantly reduced final germination, germination energy, root and shoot elongation, photosynthetic pigment accumulation, and the maximum quantum efficiency of photosystem II (Fv/Fm). It also markedly increased MDA accumulation and reduced plant height and 1000-grain weight, whereas leaf area and cob length remained comparatively stable. Similar combinations of impaired germination, inhibited seedling growth, pigment loss, oxidative imbalance, and altered antioxidant responses have been reported previously in gamma-irradiated maize and
Arabidopsis thaliana [
2,
6].
The protective response to ZnIM was clearly non-linear. Among the concentrations tested, 0.01% ZnIM produced the broadest and most consistent physiological response. This treatment restored final germination, germination energy, and root length to values statistically comparable with the non-irradiated control and produced the highest chlorophyll
a, total chlorophyll, carotenoid, and Fv/Fm values among the irradiated treatments. It also produced the greatest numerical reduction in MDA during the first week. In contrast, 0.1% ZnIM was generally less effective for germination, early growth, and photosynthetic traits but produced the lowest MDA values during the second and third weeks and the highest numerical 1000-grain weight among irradiated plants. The 0.001% treatment produced weaker and less persistent responses. Thus, increasing ZnIM concentration did not result in a proportional increase in protection. This pattern is biologically relevant because Zn supports numerous metabolic and structural processes within an appropriate physiological range, whereas excessive Zn exposure can inhibit germination, root development, photosynthesis, and protein accumulation and can promote ROS formation and lipid peroxidation in maize [
13].
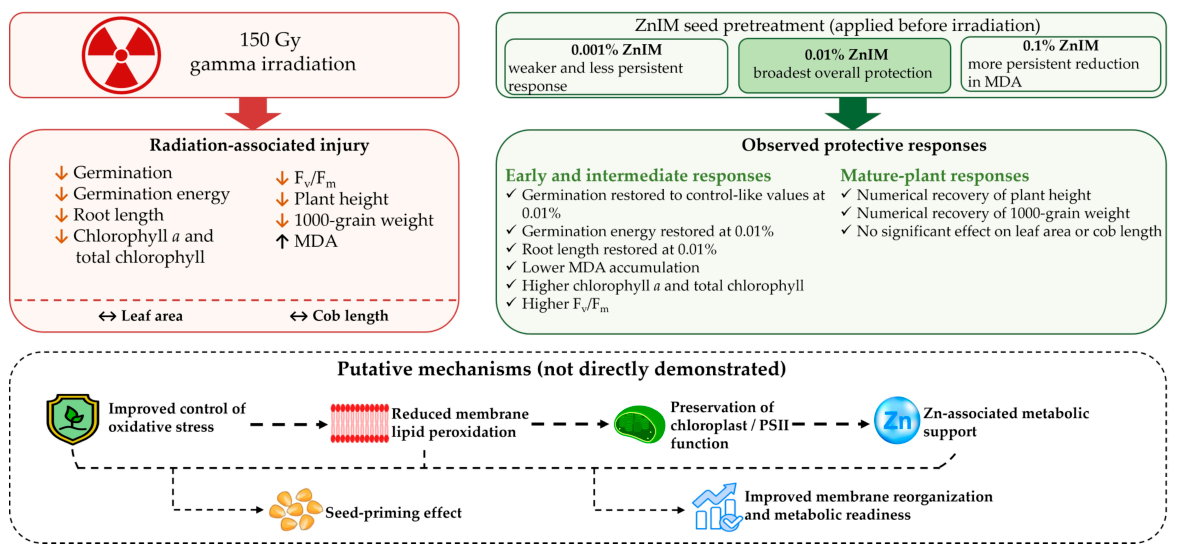
The integrated response pattern and the principal mechanistic hypotheses arising from the present study are summarized in
Figure 6. The scheme distinguishes experimentally observed responses from mechanisms that are biologically plausible but were not directly measured. The experimentally supported component of the model shows that 150 Gy irradiation was associated with impaired germination and seedling development, increased MDA accumulation, reduced photosynthetic pigment content and PSII efficiency, and persistent reductions in plant height and 1000-grain weight. ZnIM pre-treatment partially counteracted several of these responses, with 0.01% providing the broadest overall protection and 0.1% producing the most persistent reduction in MDA during later seedling development. The mechanistic pathways presented in
Figure 6 should therefore be interpreted as a working model derived from the combined physiological and biochemical evidence rather than as experimentally established causal pathways.
A physiologically coherent interpretation of these responses begins with the formation of reactive species following irradiation. Experimental studies in maize have demonstrated dose-dependent accumulation of radiation-induced free radicals accompanied by reductions in germination, seedling elongation, and photosynthetic pigment content [
6]. Studies in Lemna minor have likewise identified ROS formation and DNA damage as important early components of gamma-radiation toxicity preceding measurable effects on plant growth and reproduction [
42]. These findings provide a mechanistic framework for interpreting the coordinated biochemical and physiological disturbances observed in the present experiment.
Reactive oxygen species generated following irradiation can affect several cellular targets simultaneously. Lipidomic analysis of gamma-irradiated Arabidopsis demonstrated rapid ROS accumulation together with extensive changes in membrane glycerolipids, including pronounced degradation of chloroplast-associated lipids and alterations in membrane physical properties [
43]. Gamma irradiation has also been shown to modify antioxidant enzyme activity, chlorophyll and carotenoid content, ROS-related gene expression, and plant growth, although the direction and magnitude of these responses vary with absorbed dose, dose rate, exposure duration, species, and developmental stage [
2].
In the present study, the 2.06-fold increase in MDA during the first week provides direct evidence that enhanced membrane lipid peroxidation was an important component of the radiation response. MDA remained significantly elevated relative to the non-irradiated control during all three sampling periods, indicating that the biochemical consequences of seed irradiation persisted well into seedling development. The simultaneous reductions in chlorophyll a, total chlorophyll, and Fv/Fm are consistent with impairment of the photosynthetic apparatus. Oxidative injury to chloroplast and thylakoid membranes could disrupt pigment–protein organization and photosynthetic electron transport, thereby restricting the energy and assimilates required for cell division, organ elongation, and subsequent plant development. Such a sequence provides a physiologically coherent explanation linking increased lipid peroxidation with the observed reductions in germination, root and shoot growth, plant height, and grain mass. However, ROS concentrations, membrane permeability, chloroplast ultrastructure, and electron transport were not measured directly. The proposed sequence therefore represents an interpretation supported by the combined indicators rather than a demonstrated causal chain.
The marked reduction in MDA following ZnIM application represents the clearest biochemical evidence associated with the protective response. During the first week, all three ZnIM concentrations significantly reduced MDA relative to irradiation alone, with 0.01% producing the lowest numerical value. During subsequent development, protection became more concentration-dependent: 0.1% ZnIM produced the lowest MDA values during the second and third weeks, while the effect of 0.001% became progressively weaker and was no longer statistically significant by the third week. This temporal shift suggests that the concentration most effective during the initial oxidative response was not necessarily the concentration producing the most persistent effect.
One possible explanation for the lower MDA accumulation is improved control of cellular oxidative stress. Research on maize genotypes differing in Zn-deficiency tolerance has shown that more effective Zn homeostasis is associated with lower hydrogen peroxide accumulation, improved membrane integrity, and greater superoxide dismutase and peroxidase activities [
44]. Exogenous Zn has also been shown to strengthen antioxidant performance under other environmental stresses. In drought-stressed maize, Zn application reduced hydrogen peroxide, superoxide, and MDA accumulation while increasing the activities of superoxide dismutase, catalase, and peroxidase and maintaining chlorophyll content and gas-exchange performance [
8]. Similarly, Zn and Mn application to cold-stressed maize increased superoxide dismutase activity, reduced visible oxidative injury, and promoted root development [
27].
These findings support the hypothesis that the Zn component of ZnIM may contribute to improved redox regulation and membrane protection. Nevertheless, the present MDA data do not identify the upstream mechanism responsible for reduced lipid peroxidation. Lower MDA accumulation could result from reduced ROS formation, more efficient ROS detoxification, stabilization of membrane lipids, more effective repair of oxidized components, or a combination of these processes. Direct radical scavenging by ZnIM should therefore not be inferred because neither ROS concentrations nor radical-scavenging activity of the complex were measured. Likewise, the present results do not demonstrate activation of specific antioxidant enzymes.
A second putative mechanism involves partial preservation of the photosynthetic apparatus. Zn availability is closely associated with chlorophyll metabolism, chloroplast organization, and photosynthetic performance in maize. Transcriptomic and proteomic studies have shown that Zn deficiency reduces chlorophyll content and photosynthetic rate, alters the abundance of proteins and transcripts involved in chlorophyll biosynthesis and electron transport, disrupts thylakoid organization, and produces chloroplasts with fewer grana and less compact membrane structures [
9]. Such findings provide a physiological basis for considering adequate Zn availability as one factor potentially contributing to maintenance of chloroplast structure and function during stress.
Zn-binding proteins may also contribute indirectly to PSII stability and repair. In Arabidopsis, the zinc-finger thylakoid protein LQY1 interacts with PSII core complexes and participates in their repair and reassembly following photodamage. Plants lacking functional LQY1 exhibited lower PSII quantum efficiency, impaired electron transport, and greater ROS accumulation under high-light stress [
45]. This observation establishes a biological connection between Zn-binding proteins and maintenance of PSII function, but it does not demonstrate that externally supplied ZnIM activates LQY1-related pathways or equivalent mechanisms in maize. Such a connection should therefore be regarded only as supporting biological context.
The simultaneous increases in chlorophyll a, total chlorophyll, and Fv/Fm following treatment with 0.01% ZnIM are consistent with partial preservation of both pigment accumulation and PSII function. However, the responses were not uniform across all photosynthetic traits. Chlorophyll b and carotenoids showed only numerical recovery, and Fv/Fm remained significantly below the control despite improvement at all ZnIM concentrations. The photosynthetic response therefore represents partial rather than complete protection. Confirmation of direct chloroplast protection would require ultrastructural analysis, quantification of PSII core and antenna proteins, measurements of electron transport rate, non-photochemical quenching, photochemical quenching, and additional gas-exchange parameters.
A third mechanism incorporated into the working model in
Figure 6 is a possible seed-priming effect. ZnIM was applied to seeds before irradiation and before germination, placing the treatment at a developmental stage during which controlled hydration can initiate metabolic activation without radicle emergence. Seed priming can accelerate membrane reorganization, mitochondrial activation, enzyme synthesis, reserve mobilization, and antioxidant readiness, thereby improving subsequent germination speed, uniformity, and tolerance to environmental stress. In maize, micronutrient priming containing Zn has accelerated emergence and improved crop establishment and yield-related traits [
10]. Micronutrient seed priming has also promoted early maize growth in micronutrient-deficient soils [
11].
Under water deficit, combined Zn and glutathione priming improved maize germination, reserve metabolism, antioxidant activity, and seedling vigor [
26]. Zn- and Mn-containing seed treatments have likewise promoted root development in maize subjected to low-temperature stress, partly in association with improved nutritional status and enhanced antioxidant enzyme activity [
27]. Although these studies involved different stressors and formulations, they support the general possibility that pre-sowing Zn-containing treatments can prepare maize seeds for more effective metabolic activation under adverse conditions.
The response pattern observed in the present study is compatible with such a priming-related contribution. The clearest ZnIM effects were observed for germination, germination energy, and root elongation—traits expressed during imbibition and early seedling establishment. Improved membrane reorganization, reserve mobilization, mitochondrial activation, or antioxidant readiness could help irradiated seeds maintain the metabolic activity required for radicle emergence and root meristem function. However, these processes were not measured directly. Seed priming should therefore be considered one component of the proposed mechanistic model rather than a confirmed mode of action.
The chemical nature of the ZnIM material introduces an additional level of uncertainty. Coordination of Zn with an organic ligand could modify chemical stability, solubility, mobility, and biological availability compared with the individual components. It may also alter interactions of the material with the seed coat, cellular membranes, proteins, or endogenous ligands. The PXRD analysis demonstrated that the synthesized ZnIM material exhibited a diffraction pattern distinct from that of free imatinib, consistent with formation of a new solid-state phase. However, PXRD alone does not establish whether the intact proposed complex entered seed tissues, remained chemically stable during the 8-h aqueous treatment, or dissociated before or after uptake.
The present data likewise do not establish a specific biological role for the imatinib ligand. It is not possible to determine whether the observed responses resulted from the intact ZnIM complex, released Zn2+, free imatinib, or combined effects of dissociation products. Pharmacological effects of imatinib established in animal systems should not be extrapolated to maize without direct experimental evidence. In particular, the present study does not demonstrate direct radical-scavenging activity of imatinib or inhibition of plant protein kinases. Determining the contribution of the organic ligand will require experiments specifically designed to separate the effects of the individual components.
An important feature of the overall response is the contrast between early and mature-plant traits. ZnIM produced statistically supported effects on several early and intermediate indicators, including germination, germination energy, root length, MDA accumulation, chlorophyll a, total chlorophyll, and Fv/Fm. In contrast, increases in plant height and 1000-grain weight following 0.01% and 0.1% ZnIM were numerical and did not differ significantly from the irradiated untreated group. Leaf area and cob length were unaffected by either irradiation or ZnIM treatment.
This distinction suggests that early biochemical and physiological protection did not translate proportionally into improvement of final plant performance. A single pre-sowing treatment may exert its strongest influence during seed imbibition, germination, and early seedling establishment, whereas later vegetative development and grain filling depend on continued nutrient supply, duration of photosynthetic activity, environmental conditions, reproductive development, and assimilate transport. Zn fertilization studies have shown that effects on maize growth and yield vary substantially with application rate, timing, genotype, soil Zn status, and environmental conditions [
39,
40]. Consequently, the comparatively weak mature-plant response observed here does not invalidate the early protective effects but limits any conclusion that ZnIM improved final crop productivity.
The proposed mechanisms summarized in
Figure 6 must also be interpreted in the context of several important experimental limitations. First, the study did not include non-irradiated seeds treated with ZnIM. It is therefore not possible to determine whether the response represents specific protection against radiation injury or, at least in part, a more general growth-promoting or priming effect. Separate treatments containing free imatinib, ZnCl
2 or another Zn salt, and a non-coordinated mixture of imatinib and Zn were also absent. These controls will be necessary to determine whether coordination produces biological effects distinct from those of the individual components.
Second, uptake and chemical fate of the ZnIM material were not investigated. Measurements of total tissue Zn using ICP-MS or ICP-OES, combined with chromatographic and mass-spectrometric detection of imatinib and, where technically feasible, the intact complex, would be required to determine whether ZnIM enters the seed, dissociates during imbibition, or remains associated primarily with external seed tissues. Such analyses would also allow treatment concentration to be related to actual Zn accumulation in plant tissues.
Third, the antioxidant hypothesis requires direct biochemical testing. Future experiments should quantify hydrogen peroxide and superoxide, electrolyte leakage, protein carbonylation, reduced and oxidized glutathione, ascorbate, and the activities of major antioxidant enzymes, including superoxide dismutase, catalase, ascorbate peroxidase, guaiacol peroxidase, and glutathione reductase. Similar combinations of ROS, antioxidant-enzyme, and lipid-peroxidation measurements have been used effectively to characterize radiation responses in plants [
2,
46].
Fourth, the proposed protection of the photosynthetic apparatus requires more detailed functional and structural characterization. Measurements of net photosynthetic rate, stomatal conductance, electron transport rate, non-photochemical quenching, photochemical quenching, and the operating efficiency of PSII would provide a more complete assessment of photosynthetic function. Chloroplast microscopy and quantitative analysis of PSII proteins, including D1, D2, CP43, CP47, and light-harvesting complex components, would help determine whether ZnIM preserves PSII organization, facilitates repair, or acts primarily through indirect reduction of oxidative damage.
The possibility of direct protection against genetic damage also remains unresolved. Gamma irradiation has been experimentally associated with DNA damage, ROS formation, and activation of DNA-repair and antioxidant-response genes in plants [
42,
47]. Comet assays, micronucleus tests, chromosome-aberration analysis, and expression profiling of DNA-repair genes would therefore be valuable for determining whether ZnIM also limits radiation-induced genomic injury.
Finally, the experiment was restricted to one maize genotype, one radiation dose, three ZnIM concentrations, and four biological replicates. The temporal MDA dataset was analyzed independently within each sampling week; consequently, changes among weeks represent descriptive trends rather than statistically demonstrated temporal effects. Future experiments using factorial or repeated-measures approaches incorporating treatment, sampling time, and their interaction would provide stronger evidence for temporal and concentration-dependent differences in protection. Larger field experiments should additionally include grain yield per plant and per unit area, kernel number, harvest index, biomass accumulation, grain Zn concentration, and multi-season assessment of treatment persistence.
Taken together, the available evidence supports the working model presented in
Figure 6, in which ZnIM treatment is associated primarily with reduced secondary oxidative damage and partial preservation of membrane-associated and photosynthetic functions during early maize development. Reduced MDA accumulation represents the clearest biochemical response and is accompanied by improved germination, root elongation, chlorophyll accumulation, and PSII efficiency. The 0.01% treatment provided the broadest physiological protection across the measured traits, whereas 0.1% ZnIM produced a more persistent reduction in MDA during later seedling development. Improved redox regulation, reduced membrane lipid peroxidation, preservation of chloroplast and PSII function, Zn-associated metabolic support, and seed-priming effects constitute biologically plausible components of this model. However, none of these mechanisms was demonstrated directly, and they should therefore be regarded as testable hypotheses for future mechanistic studies rather than established modes of ZnIM action.