

Submitted:
15 March 2026
Posted:
16 March 2026
You are already at the latest version
Abstract
Antisense oligonucleotides (ASOs) are emerging therapeutic agents that modulate gene expression at the RNA level, offering distinct therapeutic advantages over conventional small-molecule drugs and biologics. By directly targeting RNA, ASOs expand the spectrum of druggable targets to include those previously considered "undruggable" and enable shorter development timelines with improved research and development efficiency. These attributes position ASOs as a highly promising platform for precision and personalized medicine. Recent advances in chemical modification strategies and delivery technologies have markedly accelerated the clinical translation. This review systematically examines the technological evolution of ASOs therapeutics, detailing their mechanisms of action, key chemical modification strategies, and advanced delivery systems. It also provides a comprehensive overview of the current global clinical landscape, including approved drugs, discontinued candidates, and ongoing clinical trials. Finally, this review discusses the major challenges facing the field and outlines future directions, with the aim of informing subsequent basic research and clinical development efforts.
Keywords:
antisense oligonucleotides
; RNA-targeted therapeutics
; chemical modification
; precision medicine
1. Introduction
RNA functions as a central mediator of cellular information flow and gene regulation. Increasing evidence suggests that both messenger RNA (mRNA) and non-coding RNA (ncRNA) contain highly structured and functionally critical elements, and that aberrations within these elements are closely linked to the pathogenesis of numerous human diseases[1]. Notably, only approximately 1.5% of the human genome encodes proteins, and up to 80% of protein-coding targets are considered "undruggable" by conventional therapeutic methods, posing a substantial challenge to drug discovery[2]. RNA-targeting therapeutics have therefore emerged as a transformative strategy, enabling access to previously inaccessible regulatory pathways and expanding the landscape of druggable targets.
Among diverse RNA-targeting strategies, oligonucleotide therapeutics have achieved remarkable clinical progress, owing to their broad target accessibility, relatively streamlined development paradigms, and controllable manufacturing costs. This class includes antisense oligonucleotides (ASOs), small interfering RNAs (siRNAs), microRNAs (miRNAs), small activating RNAs (saRNAs), and aptamers[3]. Currently, ASOs represent the most established modality among approved oligonucleotide drugs, with 14 marketed products (including subsequently withdrawn agents), outnumbering siRNAs (8) and aptamers (2), underscoring their relative maturity and leadership in clinical translation[4,5]. Continuous technological innovation, particularly iterative advances in chemical modifications and delivery platforms, has been fundamental to this success[3]. These innovations have addressed key barriers to clinical translation, including limited in vivo stability, inefficient cellular uptake, and off-target toxicity. Moreover, improved translational strategies and growing clinical validation have enabled ASOs to expanded beyond rare genetic disorders into broader chronic indications.
This review offers a systematic overview of the technological evolution of ASOs, tracing their progression from conceptual inception to contemporary clinical applications. It outlines the core mechanisms underlying ASO-mediated gene regulation, summarizes major chemical modification strategies and advanced delivery systems, and analyzes the global clinical translation landscape, including approved drugs, discontinued candidates, and ongoing clinical trials. Finally, it discusses the principal challenges facing the field and highlights future development directions, with the aim of informing both fundamental research and the advancement of next-generation clinical candidates.
2. Evolutionary History
The development of ASOs technology represents a remarkable journey in expanding druggability within the theoretical framework of the "Central Dogma". Through iterative cycles of proof-of-concept validation, periods of setbacks and stagnation, and sustained technological innovation, the field has ultimately achieved substantial clinical breakthroughs (Figure 1).
2.1. Inception and Preliminary Validation (1978–1999)
ASOs are synthetic, single-stranded nucleic acid analogs, typically ranging from 12 to 30 nucleotides in length, that selectively recognize and bind target RNA through Watson–Crick base pairing, thereby modulating gene expression[6]. The concept of the ASO was initially introduced by Paul C. Zamecnik and Mary L. Stephenson in 1978, when they demonstrated that a sequence-specific oligonucleotide complementary to Rous sarcoma virus 35S RNA could inhibit viral replication in tissue culture, establishing the theoretical foundation of the field[7,8].
Over the following two decades, first-generation chemical modifications (most notably phosphorothioate (PS) backbone substitution) were developed to overcome poor nuclease stability and suboptimal pharmacokinetic properties[9]. A milestone during this period was the 1998 approval by the U.S. Food and Drug Administration (FDA) of Fomivirsen (Vitravene) for the treatment of cytomegalovirus retinitis in AIDS patients[10]. Fomivirse was restricted to local intravitreal injection, because it failed to resolve the metabolic and toxicity challenges associated with systemic administration[11]. Its eventual withdrawal underscored the inherent limitations of first-generation ASOs technology and highlighted the need for further chemical and delivery innovations.
2.2. Setbacks and Technological Reshaping (2000–2015)
At the beginning of the 21st century, the ASOs field faced a critical trade-off between toxicity and efficacy. First-generation ASOs were limited by low target affinity, non-specific immune activation, and severe off-target toxicity, resulting in multiple Phase III trials failures and plunging the field into a "valley of Death"[12]. A pivotal turning point came with the advent of second-generation chemistries, including 2′-O-methoxyethyl (2′-MOE), together with the implementation of the chimeric "Gapmer" design strategy [13]. The 2013 FDA approval of Mipomersen (Kynamro) for the treatment of homozygous familial hypercholesterolemia reignited enthusiasm for ASOs development [14]. Although Mipomersen faced commercial setbacks due to injection-site reactions and hepatotoxicity, it provided proof of concept for the systemic reduction of liver-derived target proteins [15]. These safety concerns, in turn, catalyzed advances in precision engineering, including N-acetylgalactosamine (GalNAc)-mediated liver targeting, stereopure (chiral) synthesis, and protein-interaction profile optimization [16,17]. Additionally, the pioneering application of the Risk Evaluation and Mitigation Strategy and the granting of orphan drug designation for Mipomersen established important operational and regulatory precedents, offering a framework that has informed subsequent ASOs development [18].
2.3. Clinical Explosion and the Golden Age (2016–Present)
With the continued refinement of chemical modifications, such as locked nucleic acid (LNA) and constrained ethyl (cEt), alongside advances in delivery technologies, ASOs have entered a period of rapid clinical development [13,17]. The approval of Nusinersen (Spinraza) in 2016 marked a transformative milestone. Administered via intrathecal injection to bypass the blood–brain barrier, it provided an effectively treatment for spinal muscular atrophy, previously recognized as a leading genetic cause of infant mortality [19]. This success validated the therapeutic potential of ASOs in splice modulation and restored confidence in nucleic acid therapeutics within the pharmaceutical industry. Additionally, GalNAc conjugation also has revolutionized hepatic targeting. A new generation of ASOs, exemplified by Eplontersen and Olezarsen, has demonstrated high potency and sustained efficacy, with dosing intervals extended up to as long as six months while maintaining favorable safety profile[16,20,21]. Collectively, these advances have propelled ASOs from a niche modality focused primarily on orphan diseases to a versatile therapeutic platform with broad potential across diverse indications.
3. Mechanisms of Action
ASOs modulate gene expression through sequence-specific hybridization with target RNA[6] (Figure 2). Their action process can be conceptualized into three stages: pre-hybridization, hybridization, and post-hybridization.
3.1. Pre-hybridization: Cellular Uptake and Trafficking
Upon entering the tissue, ASOs can be passively internalized through gymnosis; however, cellular uptake predominantly relies on receptor-mediated endocytosis[22]. Cell surface receptors, such as Stabilin-1and Stabilin-2, recognize and internalize ASOs via clathrin-dependent pathways, serving as a major in vivo entry route[23,24]. In hepatocytes, the asialoglycoprotein receptor exhibits high endocytic efficiency; multivalent GalNAc ligands promote synergistic receptor engagement, induce conformational changes, and promote efficient ASO endocytosis[25].
Following endocytosis, ASOs traffic from early endosomes to late endosomes or multivesicular bodies. Only the small fraction can successfully escape into the cytoplasm or nucleus, where they exert their biological activity, making endosomal escape the principal rate-limiting step for therapeutic efficacy[26]. Intracellularly, ASOs form dynamic complexes with nucleic acid-binding proteins that regulate their nucleocytoplasmic shuttling and intracellular retention[9].
The chemical structure of ASOs determines their protein-binding properties, subcellular localization, and applicable administration routes[27]. Fully PS backbones enhance reversible binding to plasma proteins, increase nuclease resistance, prolong circulating half-life, and promote accumulation in highly perfused tissues such as the liver and kidneys following intravenous administration[28]. Conversely, mixed backbones, chimeric structures composed of phosphorothioate and phosphodiester linkages, reduce protein-binding affinity and accelerate renal clearance, making them appropriate for local administration settings where minimal systemic exposure is desired[29]. Chiral phosphorus backbones further improve target RNA binding specificity through defined spatial configuration, thereby reducing off-target effects and informing the selection of optimal administration routes[30].
3.2. Hybridization: Target RNA Recognition
Following successful intracellular trafficking to the appropriate subcellular compartments, ASOs initiate sequence-specific molecular recognition and hybridization with their target RNA[31]. To achieve effective binding, they must overcome steric hindrance imposed by complex RNA structures, such as hairpins and pseudoknots, and dynamically compete with endogenous RNA-binding proteins already associated with the transcript[32]. These proteins include spliceosomal components that regulate pre-mRNA splicing, heterogeneous nuclear ribonucleoproteins responsible for RNA transport and processing, and ribosomes engaged in translation[32,33]. The spatial accessibility of the target site, along with the hybridization kinetics, are key efficacy determinants. These factors govern binding stability, target engagement efficiency, and ultimately the magnitude and durability of the pharmacological response[34].
3.3. Post-hybridization: Functional Modulation of Target RNA
Upon formation of a stable ASO-target RNA complex, ASOs exert their effects through distinct mechanistic pathways defined by how they modulate target RNA function[35]. A major class operates via RNase H1–dependent cleavage. In this mechanism, ASOs form DNA/RNA heteroduplexes with the target transcript, thereby recruiting the endogenous endonuclease RNase H1. Activation of RNase H1 induces site-specific cleavage of phosphodiester bonds within the RNA strand, resulting in degradation of pathogenic transcripts and suppression of pathogenic protein translation[35]. Because RNase H1 is localized in both the cytoplasm and nucleus, this pathway enables the degradation of mature cytoplasmic mRNAs as well as nuclear-retained pre-mRNAs and immature transcripts, thereby broadening the spectrum of targetable RNAs[36].
In contrast, RNase H1-independent ASOs function primarily through steric hindrance. These molecules competitively bind to specifict RNA sequences and physically obstruct interactions with regulatory proteins, spliceosomes, or ribosomes[37]. Within the nucleus, splice-switching ASOs target exon–intron junctions or splicing regulatory elements to modulate alternative splicing. For example, in Duchenne muscular dystrophy, exon-skipping ASOs restore the translational reading frame, enabling the production of partially functional dystrophin[38]. In the cytoplasm, ASOs bind regulatory regions such as the 5′ untranslated region or upstream open reading frames to modulate translation, either enhancing protein synthesis by relieving inhibitory elements or suppressing initiation to reduce protein expression[39]. This steric mechanism also extends to ncRNAs, including miRNAs and long non-coding RNAs (lncRNAs), by reducing their abundance or obstructing their functional domains[3].
Beyond these classic mechanisms, several emerging strategies are under active investigation. Notably, RNA in situ editing through adenosine deaminase acting on RNA-recruiting ASOs enables precise adenosine-to-inosine conversion to correct pathogenic mutations at the RNA level without modifying genomic DNA[40]. Additionally, ASOs can form triplex structures with DNA or RNA duplexes to inhibit transcription[41], or mask RNA-binding protein recognition motifs, thereby modulating RNA splicing, stability, and translation efficiency[42]. Collectively, these expanding mechanistic modalities significantly broaden the therapeutic scope of ASOs in gene regulation and precision therapeutics.
4. Chemical Modifications
Mechanisms of action define the functional direction and efficacy of ASOs, whereas chemical modifications balance selectivity and safety, endowing the stability and druggability[43] (Figure 3). The progressive maturation of these complementary technologies has been instrumental in translating ASOs from conceptual innovation to validated clinical therapeutics.
4.1. Backbone Modifications
Backbone modifications are central to improving metabolic stability, minimizing immunogenicity, and optimizing tissue distribution, with phosphodiester (PO) linkages modification as the foundational strategy[9,35]. Among these, PS substitution, where a non-bridging phosphate oxygen is replaced by sulfur, is the most clinically established backbone modification[9]. PS chemistry enhances nuclease resistance, alters biodistribution through improved protein interactions, and preserves the ability to recruit RNase H[44]. Accordingly, the majority of approved ASOs incorporate PS linkages. The "Gapmer" structure further optimizes the therapeutic index by combining a central DNA-like "gap," which supports RNase H1–mediated cleavage, with chemically modified "wings" that enhance affinity and stability[37]. Moreover, stereoselective synthesis controlling the chirality (Sp or Rp) of PS linkages reduces backbone heterogeneity, mitigates non-specific interactions, and enhances efficacy[30,45]. Emerging non-natural linkages, such as mesyl-phosphoramidate (MsPA), phosphoryl-guanidine (PG), and boranophosphate (PB), further modulate surface charge and conformational properties, thereby improving cellular uptake while maintaining RNase H1 compatibility and reducing immune stimulation[46,47].
Another alternative strategy involves modifying the topological framework of the oligonucleotide[13]. Phosphorodiamidate morpholino oligomers (PMOs) replace the ribose ring with a morpholine moiety linked via neutral phosphorodiamidate bonds, substantially reducing non-specific protein interactions[13,38]. Operating primarily through steric blockade, PMOs are well suited for prolonged intravenous administration, as exemplified by for the treatment of Duchenne muscular dystrophy[48]. Thiophosphoramidate morpholinos (TMOs) further improve stability through sulfur or nitrogen modifications[49]. Peptide nucleic acids (PNAs) use a neutral pseudopeptide backbone that eliminates electrostatic repulsion, thereby strengthening target-binding affinity[50]. Similarly, serinol nucleic acids (SNAs), in which ribose is replaced by serinol, enable hybridization with various chiral oligonucleotides, offering additional opportunities to optimize the stability and sequence specificity[51,52].
4.2. Sugar Modifications
Sugar modifications, particularly at the 2′ position of the ribose ring or through conformational locking, substantially enhance target affinity, improve stability, and reduce toxicity[53]. Classical non-bridged 2′ modifications, such as 2′-O-methyl (2′-OMe), 2′-O-methoxyethyl (2′-MOE), and 2′-fluoro (2′-F), favor a C3′-endo sugar pucker, thereby strengthening hybridization to complementary mRNA sequences[54]. Among these, 2′-MOE, a representative of second-generation chemistry, confers enhanced nuclease stability and attenuates immunogenicity[55]. The 2′-OMe modification is synthetically accessible and well tolerated, whereas 2′-F further increases binding affinity with minimal steric hindrance, albeit with potential concerns regarding metabolite-associated toxicity[56]. The clinical success of Nusinersen (Spinraza), an 18-mer PS backbone ASO uniformly modified with 2'-MOE, exemplifies the impact of sugar chemistry optimization, enabling high-affinity binding to SMN2 pre-mRNA and pioneering splicing-modulating therapy for spinal muscular atrophy[57]. Additionally, the 2′-O-[2-(N-methylcarbamoyl) ethyl] (2′-MCE) modification demonstrates comparable activity to 2′-MOE with reduced hepatotoxicity, positioning it as a promising next-generation 2′-O-alkyl alternative[58]. Conformationally locked bridged nucleic acids (BNAs), which establish a 2' - 4' chemical bridge, have been developed to optimize ASOs hybridization affinity and structural rigidity[59]. Locked nucleic acids (LNAs), characterized by a 2′-O,4′-C-methylene bridge, increase the melting temperature by approximately 3–8°C per monomer[60]. The introduction of a methyl group to LNAs, forming constrained ethyl (cEt) derivatives, further improves the therapeutic index[61]. Ongoing efforts focus on reducing toxicity, as demonstrated by BNAP-AEO’s ability to mitigate central nervous system toxicity, and optimizing tissue distribution, with cycloalkane-incorporated BNAs enhance dosing efficiency[59,62].
For ribose-deficient backbones systems such as PMO and PNAs, limited membrane permeability and suboptimal solubility remain the key challenges, which are being addressed through modifications of side-chains, linkages, or terminals[35]. For example, arginine-rich cell-penetrating peptides promote endocytosis[63], cationic linkers create "charge-chimeric" PMOs to enhance muscle uptake[64], and lipid or GalNAc conjugates enable efficient tissue-selective biodistribution[65].
4.3. Nucleobase Modification
Unmodified CpG motifs, which are cytosine–guanine dinucleotides, activate Toll-like receptor 9 (TLR9), leading to severe influenza-like symptoms and inflammatory responses in early candidate ASOs[66]. The modification of CpG motifs with 5-methylcytosine (5-MeC) effectively mimics endogenous DNA methylation, thereby preventing innate immune activation without altering heteroduplex geometry[53]. This kind of modification is frequently employed in current clinical ASOs.
To develop shorter and more potent ASOs, heterocyclic bases are engineered to introduce additional hydrogen bonds or enhance stacking interactions. For instance, C5-propynyl substitutions (C5-propynyl-C/U) strengthen π–π stacking, thereby increasing the melting temperature[67,68]. Additionally, the G-Clamp, a tricyclic cytosine analog, forms four hydrogen bonds with guanine, allowing for the reduction in an ASO length to 10–12 nucleotides (as opposed to the conventional ~20 nucleotides) and consequently decreasing renal burden[69,70].
5. Delivery Strategies
Despite chemical modifications, ASOs’ high hydrophilicity and large molecular weight limit intrinsic transmembrane permeability, making efficient, safe, and precise delivery a critical bottleneck in ASOs developments. The common delivery strategies are shown in Figure 4.
5.1. Naked ASOs
Naked ASOs depend on their inherent physicochemical properties for in vivo distribution and cellular uptake[65]. They demonstrate efficacy in local administration but face challenges in systemic delivery. Local administration methods, such as intravitreal injection, are commonly used for ocular diseases, as evidenced by the use of Fomivirsen (Vitravene)[71]. In contrast, by the contrast early systemic administration strategies, including intravenous or subcutaneous routes, required high doses to achieve passive uptake by the reticuloendothelial system, leading to non-specific accumulation in the liver and kidneys and raising biosafety concerns, as seen with Mipomersen (Kynamro))[72]. Furthermore, systemic administration is ineffective at penetrating brain tissue due to the blood-brain barrier[73]. However, ASOs exhibit a prolonged half-life in cerebrospinal fluid, lasting several months, which facilitates extensive distribution in the spinal cord and brain[74]. Consequently, intrathecal injection of naked ASOs has become the "gold standard" for treating central nervous system diseases, as exemplified by Nusinersen (Spinraza)[74,75].
5.2. Conjugate-Based Delivery
Conjugate-based delivery attaches biologically active ligands or carriers to ASOs, thereby precisely modulating their delivery properties[23]. Ligands, such as carbohydrates, vitamins, and small molecules, are conjugated to the termini of ASOs through click chemistry or linkers, exploiting receptor-ligand interactions to facilitate tissue-specific endocytosis[23,76]. For instance, trivalent GalNAc binds to the asialoglycoprotein receptor, enhancing hepatic targeting, reducing the required dosage, and extending dosing intervals[25]. Comparative studies between Inotersen (Tegsedi) and GalNAc-conjugated Eplontersen (Wainua), (both targeting transthyretin, demonstrate that Eplontersen exhibits superior efficacy and a lower incidence of thrombocytopenia and nephrotoxicity[21]. However, the hepatocyte-specific targeting of GalNAc presents limitations for certain therapeutic applications. For example, Bepirovirsen (GSK3228836)[77,78], which is more effective than its GalNAc-conjugated counterpart (GSK3389404)[79,80], circumvents the use of GalNAc to facilitate entry into hepatocytes for viral transcript degradation and access to non-parenchymal cells for immune stimulation, thereby enhancing the treatment of hepatitis B[81].
Lipophilic moieties, such ascholesterol, palmitic acid, vitamin E, and bile acids, have been shown to enhance the pharmacokinetics and cellular uptake of ASOs[82]. Imetelstat (Rytelo), a telomerase inhibitor approved in 2024, utilizes a palmitoyl modification and a specialized phosphorothioamidate (N3′–P5′) backbone to improve exposure and uptake, thereby increasing its efficacy in treating bone marrow disease[83,84]. Studies have demonstrated that ASOs conjugated with fatty-acid can improve muscle cellular uptake and gene-silencing potency[85], while ASOs conjugated with vitamin E or cholesterol enhance tumor uptake and activity[86].
Biomacromolecules, including antibodies, peptides, and aptamers, facilitate "precise targeting" and enable penetration into deep tissues[87]. Antibody–oligonucleotide conjugates (AOCs), such as those involving anti-transferrin receptor 1(TfR1)-antibodies, enhance the crossing of the blood-brain barrier or uptake by muscle tissues[88,89]. Peptide–oligonucleotide conjugates (POCs) utilize cell-penetrating peptides or homing peptides to improve membrane translocation and facilitate endosomal escape, as demonstrated by peptide-conjugated PMO technology in the treatment of neuromuscular diseases[63,90]. Aptamers, which are structured nucleic acids that recognize cell surface receptors through spatial complementarity[91], are instrumental in guiding the delivery of drugs. A recently study shown that the gold nanoparticles conjugated with an α7/β1 integrin-targeting aptamer have been used to deliver microRNA-206 to muscle satellite cells, promoting muscle regeneration in a mouse model of Duchenne muscular dystrophy[92], which provides a potential research direction for the targeted delivery of ASOs.
5.3. Carrier-Based Delivery
In addition to conjugate-based strategies, various carrier-based delivery systems being developed to address the challenges associated with the cellular uptake of ASOs.
Lipid-based nanoparticles, which include liposomes, lipid nanoparticles, lipid nanoemulsions, solid lipid nanoparticles, and nanostructured lipid carriers, are designed to navigate physiological barriers effectively[93]. Among these, lipid nanoparticles, characterized by anionizable lipid core, are recognized as the most efficient vehicles for the delivery of small nucleic acid[94]. Solid lipid nanoparticles and nanostructured lipid carriers provide advantages such as stability and sustained release[95], while lipid nanoemulsions are particularly suitable for the solubilization of lipophilic cargo in multimodal systems[96].
Synthetic polymers such as polyethyleneimine and polylactic-co-glycolic acid, along with natural polymers like chitosan and hyaluronic acid, as well as lipid–polymer hybrid nanoparticles, facilitate the formation of polyplexes with ASOs through electrostatic interactions, thereby safeguarding them from degradation[97]. Additionally, the incorporation of stimulus-responsive modifications in the polymer side chains, such as pH or redox-responsive motifs, can potentially be employed to enhance the compartment-specific release of ASOs within cells[98].
Inorganic nanocarriers, such as mesoporous silica nanoparticles, gold nanoparticles, silver nanoparticles, and iron oxide nanoparticles, exhibit controllable properties and surface modification capabilities[99]. Mesoporous silica nanoparticles, are characterized by their ultra-high specific surface area and ordered mesoporous structures, which facilitate efficient drug loading and controlled release[100]. Gold and silver nanoparticles utilize metal-sulfur bonds or electrostatic interactions to achieve high-density loading, thereby enhancing resistance to nucleases[101]. For instance, functionalized ASO–gold nanoparticles have been used to inhibit pathogenic genes in drug-resistant bacteria, thereby restoring sensitivity to β-lactam antibiotics[102]. Iron oxide nanoparticles enable magnetically targeted delivery through external magnetic fields and serve as theranostic agents, particularly as contrast agents in magnetic resonance imaging[103]. Additionally, the surface engineering of inorganic carriers can synergistically improve cellular uptake. For instance, ASOTARI, which consists of glucose polymer-modified silica nanoparticles, is selectively internalized by bacteria via the bacterial-specific ABC sugar transporter pathway, facilitating targeted treatment of drug-resistant bacterial keratitis[104].
Biomimetic and cell-derived carriers exhibit low immunogenicity and exceptional ability to penetrate biological barriers, effectively delivering therapeutic agents by emulating endogenous biological transport mechanisms[105]. Exosomes, also known as extracellular vesicles, are natural facilitators of intercellular communication. They possess distinctive surface proteins and lipid compositions that endow them with tissue-targeting capabilities and membrane fusion potential, thereby protecting ASOs from immune clearance and aiding in endosomal escape[106]. CDK-004 (exoASO-STAT6), an exosome-mediated ASO targeting STAT6 for the treatment of hepatocellular carcinoma, was previously investigated but ultimately discontinued due to the complexity of the delivery system, as well as concerns regarding efficacy and safety[107]. Cell-membrane vesicles, which are created by coating carriers with membrane components derived from erythrocytes, leukocytes, or tumor cells, provide a "camouflage effect" that extends the circulation time of ASOs. Additionally, they exploit the chemotactic properties of the source cells to achieve targeted enrichment at sites of inflammation or tumor, thereby enhancing biocompatibility and targeting precision[108].
6. Clinical Translation Landscape
6.1 Insights from Approved Drugs
ASOs have emerged as a promising class of sequence-specific nucleic acid therapeutics, with their clinical efficacy substantiated by an increasing number of approved drugs across diverse disease areas. This overview synthesizes their key clinical breakthroughs and technological advancements to underscore their expanding role in contemporary therapy (see Table 1).
The clinical translation of ASOs began with technological exploration and regulatory validation, a foundational stage exemplified by the approval of Fomivirsen (Vitravene) during the early technological era. Administered via intravitreal injection, Fomivirsen circumvented systemic delivery risks, minimized whole-body exposure, and facilitated the monitoring of therapeutic efficacy[11]. Its success not only marked a pivotal breakthrough in the clinical application of ASOs but also provided regulatory validation for sequence-specific nucleic acid therapeutics, thereby laying the groundwork for subsequent advancements towards systemic delivery, the next critical stage in ASO evolution.
Building on the regulatory and technological foundations established by Fomivirsen, ASOs have progressed to systemic delivery, demonstrating significant advancements in the treatment of liver-related diseases. The liver's intrinsic capacity for high oligonucleotide uptake, due to its role as a major source of circulating proteins and metabolic factors, facilitates effective systemic delivery of ASOs[109]. Mipomersen (Kynamro), the first systemically administered ASO targeting APOB-100 for homozygous familial hypercholesterolemia, established safety parameters for systemic ASO delivery through its market withdrawal[76]. In contrast, Volanesorsen (Waylivra) and Olezarsen (Tryngolza), both targeting the APOC3 pathway, illustrate advancements in the platform. Notably, Olezarsen achieves a 50–60% reduction in triglycerides through monthly subcutaneous administration, while eliminating thrombocytopenia toxicity and negating the need for complex Risk Evaluation and Mitigation Strategies [20,110]. In the context of hereditary transthyretin-mediated amyloidosis, the successful approvals of Inotersen (Tegsedi) and Eplontersen (Wainua) have established ASOs as a foundational therapy for liver-derived diseases[111]. Overall, cardiovascular and metabolic disorders serve as a critical bridge for ASOs transitioning from orphan drugs to chronic disease therapeutics, paving the way for their exploration in complex areas like neurological disorders.
Building on their success in treating liver and metabolic diseases, ASOs have achieved clinical prominence in the realm of neurological disorders, an area characterized by significant unmet medical needs. This advancement is largely attributed to the sophisticated application of PMO technology and enhanced delivery methods[13]. PMO technology enhances ASO stability and target specificity in the central nervous system, enabling the approval of four ASOs—Eteplirsen (Exondys 51), Golodirsen (Vyondys 53), Viltolarsen (Viltepso), and Casimersen (Amondys 45)—for the treatment of Duchenne muscular dystrophy by modulating splicing to restore the reading frame or enhance functional transcripts[38]. Additionally, the use of intrathecal injection allows for the bypassing of the blood-brain barrier, enabling direct delivery to the central nervous system, with Nusinersen (Spinraza) serving as a benchmark for central nervous system targeted ASOs[112]. Beyond this, Tofersen (Qalsody), approved for SOD1-associated amyotrophic lateral sclerosis based on reductions in neurofilament light chain rather than solely clinical survival, has established a new paradigm for the accelerated approval applicable to other disease areas, including oncology[113].
Leveraging technological advances and approval paradigms from neurological and metabolic diseases, ASOs have expanded into oncology with innovative applications that extend their druggable space beyond traditional RNA expression modulation. Imetelstat (Rytelo), the first oligonucleotide telomerase inhibitor approved for oncological use, addresses a critical unmet need in patients with lower- to intermediate-risk, transfusion-dependent myelodysplastic syndromes [114]. Unlike classical PS-gapmer ASOs, which primarily focus on modulating RNA expression, Imetelstat binds to the template region of the telomerase RNA component, directly inhibiting enzymatic activity. This action results in telomere shortening and apoptosis of malignant clones, classifying it as a sequence-specific RNA-targeting oligonucleotides[115]. Its approval not only expands the ASO therapeutic landscape to include functional inhibition of RNA–protein complexes but also paves the way for ASO-based cancer therapies, potentially extending their application to areas such as inflammation and immunotherapy.
In conjunction with their expansion into oncology, ASOs have made significant strides in the fields of inflammation and immunotherapy—representing the latest frontier in their clinical development. This progress is marked by a strategic transition from acute symptom control to long-acting prevention, thereby enhancing patient adherence and disease management. A notable example of this shift is Donidalorsen (Dawnzera), which received approval in 2025 for the prophylaxis of hereditary angioedema in patients aged 12 years and older. Donidalorsen offers flexible subcutaneous dosing options (every 4 or 8 weeks) and reduces frequency and severity of attacks by reducing plasma prekallikrein levels to inhibit the overactivation of bradykinin pathway[116]. Its approval underscores the role of ASOs in sustainable disease management and broadens their clinical application scenarios. Collectively, these advancements across metabolic, neurological, oncologic, and inflammatory diseases reflect the progressive evolution of ASO technology. This evolution raises important questions regarding the logical sequence of their clinical development, which will be analyzed in the subsequent section.
6.2. Lessons from Failed Attempts
The clinical application of ASOs is accompanied by numerous challenges. Analyzing unsuccessful candidates offers valuable insights for future research and development efforts. To highlight these critical obstacles and derive actionable lessons, this discussion focuses on representative examples. A comprehensive summary of drugs that did not succeed in clinical trials is presented in Table 2.
One major challenge in the clinical application of ASOs is the imbalance between risk and benefit, which can lead to the discontinuation of products if long-term systemic toxicity or unacceptable safety signals arise, making risk management impractical. For example, (Kynamro) carried a Boxed Warning and required Risk Evaluation and Mitigation Strategies due to the risks of elevated transaminases and hepatic steatosis risks, and it was ultimately withdrawn from the market in 2019, only five years after receiving approval, due to severe hepatotoxicity[18]. Similarly, Vupanorsen, which targets ANGPTL3, exemplifies a mid-stage termination resulting from an unfavorable risk-benefit profile. Pfizer and Ionis discontinued the program in 2022 because the Phase IIb lipid-lowering efficacy was insufficient to counterbalance emerging concerns about hepatic steatosis[117]. Additionally, SRP-5051 (Vesleteplirsen), designed to improve the uptake of PMOs in neuromuscular diseases through conjugation with an arginine-rich cell-penetrating peptide, demonstrated greater potency than first-generation PMOs. However, it led to severe hypomagnesemia and the renal tubular toxicity due to renal accumulation of the cationic peptide, prompting Sarepta to announce the discontinuation of exon 51-skipping therapy for Duchenne muscular dystrophy[118]. These cases highlight that ASOs are not inherently unsafe; rather, the therapeutic window is collectively influenced by factors such as the chemical backbone, sequence characteristics, dosage exposure, and the risk profile of the patient population. Like the FDA's 2024 guidance on “Clinical pharmacology considerations for the development of oligonucleotide therapeutics” emphasizes systematic assessment of immunogenicity, hepatic and renal impairments, and drug–drug interactions[119].
Another critical hurdle is the failure to establish meaningful efficacy endpoints, particularly in oncology and other complex systemic diseases. Factors such as tissue heterogeneity, compensatory pathways, and the contexts of combination therapy frequently impede the translation of single-target knockdown into meaningful clinical benefits, particularly as the standard of care continues to evolve[120]. Clinical trial designs must address three critical questions: "What is the incremental benefit?", "Who benefits?" and "How does it complement existing therapies?" Without clear answers to these questions, Phase III programs may be terminated due to negative primary endpoints or futility, even when early molecular signals are positive[121].A notable example is Custirsen (OGX-011), which targets Clusterin in prostate cancer. Phase III clinical trials evaluating Custirsen in combination with docetaxel and prednisone for metastatic castration-resistant prostate cancer failed to demonstrate a benefit in overall survival, as was similarly observed in a subsequent study involving cabazitaxel[122,123]. Casimersen, which received approval based on the surrogate endpoint of increased dystrophin expression, reported that its post-marketing confirmatory Phase III trial (NCT02500381) failed to meet the primary clinical endpoints[124], which underscores the uncertainty of translating surrogate endpoints into long-term clinical benefits. Sarepta is currently engaged in discussions with the FDA regarding potential withdrawal or alternative supporting evidence of Casimersen[125]. The principal challenge for ASOs in complex diseases may not be the binding to target RNA, but rather achieving adequate effective exposure and effect size to impact survival or remission endpoints. Therefore, current development strategies should prioritize biomarker-driven patient stratification, combination therapies, and innovations in delivery methods.
An often underappreciated yet equally significant challenge in therapeutic development is the discrepancy between the site of delivery and the effect at the clinical endpoint. Successful delivery to the target organ does not guarantee access to cellular compartments essential for clinical endpoints. For instance, Sepofarsen, developed by ProQR for targeting CEP290 in Leber Congenital Amaurosis 10, failed to meet the primary endpoint of improved Best Corrected Visual Acuity in a pivotal Phase II/III trial[126]. In-depth analysis revealed that although Sepofarsen restored full-length CEP290 protein at the molecular level, the photoreceptor cell structures in patients with advanced disease stages had undergone irreversible degeneration, and simultaneously the concentrations of the drug in the central macular fovea may have been insufficient[127]. Similarly, Tominersen (RG6042) developed for Huntington’s disease and targeting the huntingtin protein, demonstrated reductions in cerebrospinal fluid huntingtin protein levels in Phase I/II trials[128]. However, the Phase III was terminated prematurely due to a lack of clinical benefit and adverse trends in the high-dose cohorts[129]. A critical factor in this outcome was Tominersen’s non-selective knockdown of both mutant and wild-type huntingtin proteins, with the latter being essential for neuronal survival[130]. These failures indicate that even with effective administration routes, functional endpoints may be limited by disease stage, exposure variability, and irreversible tissue damage.
In addition to scientific and regulatory challenges, the limited commercial viability of ASOs can impede their clinical application, even when these drugs possess a robust mechanistic rationale and demonstrated efficacy. Changes in the therapeutic landscape, diminished patient demand, or the emergence of superior treatment modalities can render certain drugs clinically unnecessary. For instance, Fomivirsen (Vitravene), a landmark in pharmaceutical history, was voluntarily withdrawn from the European market in 2002 due to "commercial reasons rather than safety concerns[131]”, primarily because the advent of highly active antiretroviral therapy , which drastically reduced cytomegalovirus retinitis incidence[18]. The clinical application of ASOs is thus influenced not only by scientific and regulatory factors but also by epidemiology of diseases, the evolution of treatment landscapes, and commercial accessibility, particularly in infectious diseases, ophthalmology, and rare diseases.
6.3. Trends in the Clinical Pipeline
ASOs applications are expanding across neurological, neuromuscular, ophthalmic, respiratory, renal, inflammatory-immune, infectious, and oncological indications. Here, only representative examples are discussed; a summary of investigational drugs currently in clinical trials is provided in Table 3.
Most Phase III programs focus on indications with well-established regulatory and clinical pathways, aligning with recent approvals (e.g., Olezarsen, Eplontersen, Donidalorsen, Tofersen, and Imetelstat). These candidates target three main areas: (i) liver-derived targets in cardiovascular or metabolic diseases and immune–inflammatory disorders; (ii) neurological diseases amenable to intrathecal injection; and (iii) infectious diseases with clear virologic endpoints or attack-frequency outcomes.
Pelacarsen (TQJ230; targeting Lp[a]) represents the largest global ASOs clinical trial to date to date, its cardiovascular outcomes trial readout will determine ASOs’ potential to penetrate the mainstream cardiovascular pharmacotherapy market[132]. ION582 (BIIB121) and GTX-102 (Apazunersen) exemplify "gene activation" strategy, they target UBE3A silencing regions to "unsilence" the paternal UBE3A gene to address the root cause of Angelman syndrome through shifting from “replacement” to “restorative” therapy[133]. Additionally, competition between Bepirovirsen (GSK3228836) and AHB-137 underscores that the unique clinical value of dual mechanism (target transcript degradation plus immune activation) in complex immune microenvironments of hepatitis B therapy[134].
Phase II trials serve as the primary arena for ASOs targets validation and platform iteration. Trabedersen (AP 12009; OT-101) , initially terminated in glioma setting due to insufficient clinical benefit[135], was repurposed as a potent TGF-β2 inhibitor following the identification of TGF-β as a key driver of PD-1 blockade resistance[136], and Oncotelic is now pursuing regulatory approval for OT-101 for the treatment of pancreatic and lung cancer[137]. In the neuromuscular diseases, WVE-N531 (Exon 53 skipping therapy) uses PN chemistry stereochemical modifications to optimize pharmacology, targeting muscle satellite cells to promote myofiber regeneration and achieving substantial dystrophin restoration without carriers[30]. Learning from Tominersen, WVE-003 targets the mHTT SNP3 locus for allele-selective degradation in HD, preserving wtHTT while silencing mutant protein, and is poised to initiate pivotal Phase III trials[128].
Early-stage trials feature diverse delivery formats and exploratory mechanisms. DYNE-251 (exon 51) from Dyne Therapeutics and AOC-1044 (exon 44) from Avidity use TfR1 antibody conjugation on PMO backbones for active muscle cell transport, with early data showing superior exon-skipping efficiency and protein restoration compared to unconjugated PMOs[138]. In oncology, developed BP1002 (L-Bcl-2) by encapsulating Bcl-2 antisense sequences in neutral-charged liposomes (Lipobilisome), completing dose escalation with preliminary efficacy signals[139]. For bacterial infections, ASOTARI uses a “Trojan horse” strategy via bacteria-specific ABC sugar transporters, improving gene-silencing efficiency and in vivo antibacterial activity for drug-resistant pathogens treatment[104]. In neurological disease, central nervous system indications are expanding to rare genetic disorders (e.g., Pelizaeus–Merzbacher Disease, Creutzfeldt-Jakob Disease, and Epileptic Encephalopathy), while for Alzheimer’s disease and Amyotrophic Lateral Sclerosis, research focuses on mechanism refinement and delivery optimization[140].
Beyond clinical-stage candidates, ASOs hold significant translational potential in other disease areas, particularly antifungal therapy[65,141]. Studies have shown that 2′-O-Me and LNA-gapmer ASOs can inhibit EFG1, a Candida albicans virulence transcriptional factor, suppressing hyphal formation, biofilms formation and virulence in Galleria mellonella infection models[142]. Multi-target strategies targeting virulence pathways regulatory nodes (e.g., RAS1 and RIM101) have also emerged, with combined 2′-OMe ASOs enhancing hyphal formation control[143]. A recent study constructed a functionalized nanoconstruct (FTNx) to silence FKS1 (β-1,3-glucan synthase) and CHS3 (chitin synthase), key fungal cell-wall biosynthesis genes, achieving synergistic inhibition in vitro and improved survival in a murine disseminated candidiasis model[144]. Despite challenges in fungal cell wall penetration, endocytosis, and intracellular transport, ASOs therapy holds promise as an adjunct to traditional antifungal through multi-targeting, higher-affinity backbones, and enhanced delivery systems.
Due to the highly programmable nature of sequence design, ASOs are ideal for individualized precision therapy, enabling direct translation of genetic sequencing data into drug synthesis[145]. Milasen, a landmark in gene therapy and individualized medicine (N-of-1 trials), completed the entire process from diagnosis to dosing in one year, successfully correcting a rare splicing mutation and alleviating epileptic symptoms[146]. This breakthrough catalyzed the establishment of the n-Lorem Foundation, dedicated to developing therapies for ultra-rare diseases and promoted regulatory reforms for adaptive approval and rapid-response mechanisms[147] (N-of-1 of ASOs therapy initiated by the n-Lorem Foundation are summarized in Table 4). The evolution of the ASOs field is driving a paradigm shift from “one-size-fits-all” to personalized medicine.
7. Challenges and Perspectives
7.1 Challenges
Despite the commercial success of ASOs therapeutics in treating specific diseases, their expansion to broader therapeutic indications remains hindered by multiple interconnected challenges. These bottlenecks primarily revolve around bioavailability limitations, safety thresholds optimization, and the lag in clinical evaluation frameworks, all of which demand targeted innovations to unlock the full potential of ASO-based therapies[3,18].
Delivery efficiency persists as the primary rate-limiting factor for ASOs efficacy. Although hepatocyte-targeted therapies with GalNAc conjugation have achieved substantial success, macromolecular nucleic acids still face formidable biological barriers in extrahepatic targeted diseases[76]. The blood-brain barrier remains a major obstacle for central nervous system indications, restricting effective brain tissue penetration despite advances in intrathecal delivery[73]. Additionally, low endosomal escape rates limit cytosolic or nuclear access, while microbial cell wall penetration poses unique challenges for anti-infective applications[26]. These delivery hurdles collectively result in suboptimal target engagement and require excessive dosing, exacerbating safety concerns.
Balancing potency and toxicity represent another critical challenge. Ultra-high-affinity chemistries (e.g., LNA, cEt) enhance target binding but simultaneously increase the risk of off-target hybridization with homologous transcripts, leading to unintended gene silencing or cellular dysfunction[13]. Chemical modifications can significantly improve ASOs pharmacokinetics, while they are prone to induce off-target effects and adverse events, including thrombocytopenia, hepatorenal toxicity, and immune-inflammatory responses[65].
The disconnect between preclinical models, surrogate biomarkers, and clinical outcomes magnifies development risk. For example, in Duchenne Muscular Dystrophy, increased dystrophin expression—used as a surrogate endpoint for approval—has not consistently translated to functional improvements in long-term clinical trials[38,125]. This gap highlights the need for more predictive biomarkers and clinical evaluation frameworks that better align molecular effects with patient-centric outcomes (e.g., mobility, quality of life, survival)[148]. Additionally, the high cost of ASOs development and manufacturing—exacerbated by the need for personalized or ultra-rare disease therapies—raises accessibility concerns, particularly for patients in resource-limited settings[147].
7.2. Future Directions
To address these challenges, future research will focus on three interconnected pillars: innovative delivery systems, precision engineering of ASOs molecules, and refined clinical development strategies. Advancements in delivery technology will prioritize tissue-specific targeting and enhanced transmembrane transport. For central nervous system disorders, novel strategies—such as the antibody–oligonucleotide conjugates (AOCs) targeting blood-brain barrier transport receptors (e.g., TfR1) or stimulus-responsive nanocarriers—aim to improve brain parenchymal penetration and cellular uptake[140]. For non-hepatic peripheral tissues (e.g., muscle, kidney), peptide conjugation (e.g., CPPs) and biomimetic carriers (e.g., exosomes, cell membrane vesicles) offer promising avenues to overcome endosomal barriers and reduce off-target accumulation[105]. Small-molecule endosomal escape enhancers, which disrupt endosomal membranes without inducing cytotoxicity, are also being explored to boost intracellular ASO bioavailability[87].
Precision engineering of ASOs will focus on optimizing specificity, stability, and safety. Stereopure synthesis—controlling the chiral configuration of PS linkages—reduces product heterogeneity and non-specific protein interactions, thereby narrowing the therapeutic window[30]. Allele-selective ASOs, designed to target mutant transcripts while sparing wild-type alleles (e.g., WVE-003 for Huntington’s disease), mitigate on-target toxicity associated with non-selective gene silencing[130]. Additionally, next-generation chemical modifications (e.g., 2′-MCE, BNAP-AEO) aim to maintain high binding affinity while minimizing hepatotoxicity and immunogenicity, expanding the applicability of ASOs to chronic disease populations requiring long-term treatment[3,43].
Refined clinical development strategies will emphasize biomarker-driven patient stratification and adaptive trial designs. Integrating transcriptomic and genomic data will enable the identification of patient subgroups most likely to benefit from ASOs therapy, reducing trial size and improving success rates[149]. For complex diseases (e.g., cancer, hepatitis B), combination therapies—pairing ASOs with immune checkpoint inhibitors, small molecules, or other nucleic acid therapeutics—will leverage synergistic mechanisms to overcome compensatory pathways and enhance therapeutic efficacy[109,120]. Furthermore, regulatory frameworks for personalized ASOs (e.g., N-of-1 trials for ultra-rare diseases) will continue to evolve, streamlining approval pathways while ensuring safety and efficacy[147].
As these innovations mature, ASOs therapeutics are poised to evolve from a niche orphan drug platform to the "third pillar" of pharmacotherapy—complementing small molecules and biologics. The expansion of ASOs to common diseases (e.g., cardiovascular disorders, neurodegenerative diseases) will be driven by large-scale clinical trials (e.g., Pelacarsen for Lp[a]-mediated atherosclerosis[132]) and the validation of dual-mechanism strategies (e.g., Bepirovirsen for hepatitis B, combining transcript degradation and immune activation[134]). Additionally, the emergence of RNA editing ASOs (AIMers[150]) and gene activation strategies (e.g., for Angelman syndrome) will extend ASOs applications beyond gene silencing to precise transcript correction and restoration, addressing the root cause of genetic diseases without altering genomic DNA. In summary, while significant challenges remain, the continuous refinement of chemical modifications, delivery systems, and clinical trial designs will unlock the full therapeutic potential of ASOs. By addressing unmet medical needs across rare and common diseases, ASOs are positioned to transform the landscape of precision medicine and improve outcomes for countless patients worldwide.
Author Contributions
writing—original draft preparation, L.X., H.Z., B.J., Y.J., and H.L.; writing—review and editing, L.X., H.Z., B.J., Y.J., and H.L.; visualization, L.X.; supervision, Y.J., and H.L.; project administration, Y.J., and H.L.; funding acquisition, H.L. All authors have read and agreed to the published version of the manuscript.
Funding
This study received financial support from the National Natural Science Foundation of China (No. 82574464).
Institutional Review Board Statement
Not applicable
Informed Consent Statement
Not applicable.
Data Availability Statement
No new data were created.
Conflicts of Interest
The authors declare no conflicts of interest.
Abbreviations
The following abbreviations are used in this manuscript:
| ASOs | Antisense oligonucleotides |
| mRNA | messenger RNA |
| ncRNA | non-coding RNA |
| siRNAs | small interfering RNAs |
| miRNAs | microRNAs |
| saRNAs | small activating RNAs |
| PS | phosphorothioate |
| FDA | Food and Drug Administration |
| 2′-MOE | 2′-O-methoxyethyl |
| GalNAc | N-acetylgalactosamine |
References
- K.D. Warner, C.E. Hajdin, K.M. Weeks, Principles for targeting RNA with drug-like small molecules, Nat Rev Drug Discov 17(8) (2018) 547-558. [CrossRef]
- Z. Cai, H. Ma, F. Ye, D. Lei, Z. Deng, Y. Li, R. Gu, H. Wen, Discovery of RNA-Targeting Small Molecules: Challenges and Future Directions, MedComm (2020) 6(9) (2025) e70342. [CrossRef]
- M. Liu, Y. Wang, Y. Zhang, D. Hu, L. Tang, B. Zhou, L. Yang, Landscape of small nucleic acid therapeutics: moving from the bench to the clinic as next-generation medicines, Signal Transduct Target Ther 10(1) (2025) 73. [CrossRef]
- C.M. Ballantyne, S. Vasas, M. Azizad, P. Clifton, R.S. Rosenson, T. Chang, S. Melquist, R. Zhou, M. Mushin, N.J. Leeper, J. Hellawell, D. Gaudet, Plozasiran, an RNA Interference Agent Targeting APOC3, for Mixed Hyperlipidemia, N Engl J Med 391(10) (2024) 899-912. [CrossRef]
- A. Mullard, FDA approves anti-prekallikrein drug for hereditary angioedema, Nat Rev Drug Discov 24(10) (2025) 732. [CrossRef]
- C.F. Bennett, Therapeutic Antisense Oligonucleotides Are Coming of Age, Annu Rev Med 70 (2019) 307-321. [CrossRef]
- P.C. Zamecnik, M.L. Stephenson, Inhibition of Rous sarcoma virus replication and cell transformation by a specific oligodeoxynucleotide, Proc Natl Acad Sci U S A 75(1) (1978) 280-4. [CrossRef]
- M.L. Stephenson, P.C. Zamecnik, Inhibition of Rous sarcoma viral RNA translation by a specific oligodeoxyribonucleotide, Proc Natl Acad Sci U S A 75(1) (1978) 285-8. [CrossRef]
- S.T. Crooke, T.A. Vickers, X.H. Liang, Phosphorothioate modified oligonucleotide-protein interactions, Nucleic Acids Res 48(10) (2020) 5235-5253. [CrossRef]
- M.D. de Smet, C.J. Meenken, G.J. van den Horn, Fomivirsen - a phosphorothioate oligonucleotide for the treatment of CMV retinitis, Ocul Immunol Inflamm 7(3-4) (1999) 189-98. [CrossRef]
- R.S. Geary, S.P. Henry, L.R. Grillone, Fomivirsen: clinical pharmacology and potential drug interactions, Clin Pharmacokinet 41(4) (2002) 255-60.
- P.H. Hagedorn, B.R. Hansen, T. Koch, M. Lindow, Managing the sequence-specificity of antisense oligonucleotides in drug discovery, Nucleic Acids Res 45(5) (2017) 2262-2282. [CrossRef]
- M. Egli, M. Manoharan, Chemistry, structure and function of approved oligonucleotide therapeutics, Nucleic Acids Res 51(6) (2023) 2529-2573. [CrossRef]
- P. Hair, F. Cameron, K. McKeage, Mipomersen sodium: first global approval, Drugs 73(5) (2013) 487-93. [CrossRef]
- D.J. Blom, F.J. Raal, R.D. Santos, A.D. Marais, Lomitapide and Mipomersen-Inhibiting Microsomal Triglyceride Transfer Protein (MTP) and apoB100 Synthesis, Curr Atheroscler Rep 21(12) (2019) 48. [CrossRef]
- K. Paunovska, D. Loughrey, J.E. Dahlman, Drug delivery systems for RNA therapeutics, Nat Rev Genet 23(5) (2022) 265-280. [CrossRef]
- R. Obexer, M. Nassir, E.R. Moody, P.S. Baran, S.L. Lovelock, Modern approaches to therapeutic oligonucleotide manufacturing, Science 384(6692) (2024) eadl4015. [CrossRef]
- F. Alhamadani, K. Zhang, R. Parikh, H. Wu, T.P. Rasmussen, R. Bahal, X.B. Zhong, J.E. Manautou, Adverse Drug Reactions and Toxicity of the Food and Drug Administration-Approved Antisense Oligonucleotide Drugs, Drug Metab Dispos 50(6) (2022) 879-887. [CrossRef]
- E. Mercuri, B.T. Darras, C.A. Chiriboga, J.W. Day, C. Campbell, A.M. Connolly, S.T. Iannaccone, J. Kirschner, N.L. Kuntz, K. Saito, P.B. Shieh, M. Tulinius, E.S. Mazzone, J. Montes, K.M. Bishop, Q. Yang, R. Foster, S. Gheuens, C.F. Bennett, W. Farwell, E. Schneider, D.C. De Vivo, R.S. Finkel, Nusinersen versus Sham Control in Later-Onset Spinal Muscular Atrophy, N Engl J Med 378(7) (2018) 625-635. [CrossRef]
- E.S.G. Stroes, V.J. Alexander, E. Karwatowska-Prokopczuk, R.A. Hegele, M. Arca, C.M. Ballantyne, H. Soran, T.A. Prohaska, S. Xia, H.N. Ginsberg, J.L. Witztum, S. Tsimikas, Olezarsen, Acute Pancreatitis, and Familial Chylomicronemia Syndrome, N Engl J Med 390(19) (2024) 1781-1792.
- T. Coelho, W. Marques, Jr., N.R. Dasgupta, C.C. Chao, Y. Parman, M.C. França, Jr., Y.C. Guo, J. Wixner, L.S. Ro, C.R. Calandra, P.A. Kowacs, J.L. Berk, L. Obici, F.A. Barroso, M. Weiler, I. Conceição, S.W. Jung, G. Buchele, M. Brambatti, J. Chen, S.G. Hughes, E. Schneider, N.J. Viney, A. Masri, M.R. Gertz, Y. Ando, J.D. Gillmore, S. Khella, P.J.B. Dyck, M. Waddington Cruz, Eplontersen for Hereditary Transthyretin Amyloidosis With Polyneuropathy, Jama 330(15) (2023) 1448-1458. [CrossRef]
- R.L. Juliano, The delivery of therapeutic oligonucleotides, Nucleic Acids Res 44(14) (2016) 6518-48.
- V. Kumar, W.B. Turnbull, Targeted delivery of oligonucleotides using multivalent protein-carbohydrate interactions, Chem Soc Rev 52(4) (2023) 1273-1287. [CrossRef]
- C.M. Miller, A.J. Donner, E.E. Blank, A.W. Egger, B.M. Kellar, M.E. Østergaard, P.P. Seth, E.N. Harris, Stabilin-1 and Stabilin-2 are specific receptors for the cellular internalization of phosphorothioate-modified antisense oligonucleotides (ASOs) in the liver, Nucleic Acids Res 44(6) (2016) 2782-94. [CrossRef]
- A.J. Debacker, J. Voutila, M. Catley, D. Blakey, N. Habib, Delivery of Oligonucleotides to the Liver with GalNAc: From Research to Registered Therapeutic Drug, Mol Ther 28(8) (2020) 1759-1771. [CrossRef]
- S.F. Dowdy, Endosomal escape of RNA therapeutics: How do we solve this rate-limiting problem?, Rna 29(4) (2023) 396-401. [CrossRef]
- X.H. Liang, H. Sun, W. Shen, S.T. Crooke, Identification and characterization of intracellular proteins that bind oligonucleotides with phosphorothioate linkages, Nucleic Acids Res 43(5) (2015) 2927-45. [CrossRef]
- E. Bäckström, A. Bonetti, P. Johnsson, S. Öhlin, A. Dahlén, P. Andersson, S. Andersson, P. Gennemark, Tissue pharmacokinetics of antisense oligonucleotides, Mol Ther Nucleic Acids 35(1) (2024) 102133. [CrossRef]
- B.T. Le, S. Chen, R.N. Veedu, Rational Design of Chimeric Antisense Oligonucleotides on a Mixed PO-PS Backbone for Splice-Switching Applications, Biomolecules 14(7) (2024). [CrossRef]
- N. Iwamoto, D.C.D. Butler, N. Svrzikapa, S. Mohapatra, I. Zlatev, D.W.Y. Sah, Meena, S.M. Standley, G. Lu, L.H. Apponi, M. Frank-Kamenetsky, J.J. Zhang, C. Vargeese, G.L. Verdine, Control of phosphorothioate stereochemistry substantially increases the efficacy of antisense oligonucleotides, Nat Biotechnol 35(9) (2017) 845-851. [CrossRef]
- R.S. Geary, D. Norris, R. Yu, C.F. Bennett, Pharmacokinetics, biodistribution and cell uptake of antisense oligonucleotides, Adv Drug Deliv Rev 87 (2015) 46-51. [CrossRef]
- T.A. Vickers, J.R. Wyatt, S.M. Freier, Effects of RNA secondary structure on cellular antisense activity, Nucleic Acids Res 28(6) (2000) 1340-7. [CrossRef]
- M.E. Rogalska, E. Mancini, S. Bonnal, A. Gohr, B.M. Dunyak, N. Arecco, P.G. Smith, F.H. Vaillancourt, J. Valcárcel, Transcriptome-wide splicing network reveals specialized regulatory functions of the core spliceosome, Science 386(6721) (2024) 551-560. [CrossRef]
- C. Terada, K. Oh, R. Tsubaki, B. Chan, N. Aibara, K. Ohyama, M.A. Shibata, T. Wada, M. Harada-Shiba, A. Yamayoshi, T. Yamamoto, Dynamic and static control of the off-target interactions of antisense oligonucleotides using toehold chemistry, Nat Commun 14(1) (2023) 7972. [CrossRef]
- X. Shen, D.R. Corey, Chemistry, mechanism and clinical status of antisense oligonucleotides and duplex RNAs, Nucleic Acids Res 46(4) (2018) 1584-1600. [CrossRef]
- X.H. Liang, H. Sun, J.G. Nichols, S.T. Crooke, RNase H1-Dependent Antisense Oligonucleotides Are Robustly Active in Directing RNA Cleavage in Both the Cytoplasm and the Nucleus, Mol Ther 25(9) (2017) 2075-2092. [CrossRef]
- J. Scharner, I. Aznarez, Clinical Applications of Single-Stranded Oligonucleotides: Current Landscape of Approved and In-Development Therapeutics, Mol Ther 29(2) (2021) 540-554. [CrossRef]
- L. Torres-Masjoan, S. Aguti, H. Zhou, F. Muntoni, Clinical applications of exon-skipping antisense oligonucleotides in neuromuscular diseases, Mol Ther 33(6) (2025) 2689-2704. [CrossRef]
- X.H. Liang, W. Shen, H. Sun, M.T. Migawa, T.A. Vickers, S.T. Crooke, Translation efficiency of mRNAs is increased by antisense oligonucleotides targeting upstream open reading frames, Nat Biotechnol 34(8) (2016) 875-80. [CrossRef]
- T. Merkle, S. Merz, P. Reautschnig, A. Blaha, Q. Li, P. Vogel, J. Wettengel, J.B. Li, T. Stafforst, Precise RNA editing by recruiting endogenous ADARs with antisense oligonucleotides, Nat Biotechnol 37(2) (2019) 133-138. [CrossRef]
- V. Genna, G. Portella, A. Sala, M. Terrazas, I. Serrano-Chacón, J. González, N. Villegas, L. Mateo, C. Castellazzi, M. Labrador, A. Aviño, A. Hospital, A. Gandioso, P. Aloy, I. Brun-Heath, C. Gonzalez, R. Eritja, M. Orozco, Systematic study of hybrid triplex topology and stability suggests a general triplex-mediated regulatory mechanism, Nucleic Acids Res 53(5) (2025). [CrossRef]
- A.M. Vanderplow, G.E. Dodis, Y. Rhee, J.J. Cikowski, S. Gonzalez, M.L. Smith, R.G. Gogliotti, Site-blocking antisense oligonucleotides as a mechanism to fine-tune MeCP2 expression, Rna 30(12) (2024) 1554-1571. [CrossRef]
- J. Bhamra, M. Krishna, G. Samaan, S. Pattanayak, S. Mukhopadhyay, Toxicity of Antisense Oligonucleotides is Determined by the Synergistic Interplay of Chemical Modifications and Nucleotide Sequences, Not by Either Factor Alone, Chembiochem 26(20) (2025) e202500584. [CrossRef]
- C.R. Hofman, D.R. Corey, Targeting RNA with synthetic oligonucleotides: Clinical success invites new challenges, Cell Chem Biol 31(1) (2024) 125-138. [CrossRef]
- P. Kandasamy, G. McClorey, M. Shimizu, N. Kothari, R. Alam, N. Iwamoto, J. Kumarasamy, G.R. Bommineni, A. Bezigian, O. Chivatakarn, D.C.D. Butler, M. Byrne, K. Chwalenia, K.E. Davies, J. Desai, J.D. Shelke, A.F. Durbin, R. Ellerington, B. Edwards, J. Godfrey, A. Hoss, F. Liu, K. Longo, G. Lu, S. Marappan, J. Oieni, I.H. Paik, E.P. Estabrook, C. Shivalila, M. Tischbein, T. Kawamoto, C. Rinaldi, J. Rajão-Saraiva, S. Tripathi, H. Yang, Y. Yin, X. Zhao, C. Zhou, J. Zhang, L. Apponi, M.J.A. Wood, C. Vargeese, Control of backbone chemistry and chirality boost oligonucleotide splice switching activity, Nucleic Acids Res 50(10) (2022) 5443-5466. [CrossRef]
- Y. Takahashi, K. Sato, T. Wada, Solid-Phase Synthesis of Boranophosphate/Phosphorothioate/Phosphate Chimeric Oligonucleotides and Their Potential as Antisense Oligonucleotides, J Org Chem 87(6) (2022) 3895-3909. [CrossRef]
- Patutina, S.K. Gaponova Miroshnichenko, A.V. Sen'kova, I.A. Savin, D.V. Gladkikh, E.A. Burakova, A.A. Fokina, M.A. Maslov, E.V. Shmendel, M.J.A. Wood, V.V. Vlassov, S. Altman, D.A. Stetsenko, M.A. Zenkova, Mesyl phosphoramidate backbone modified antisense oligonucleotides targeting miR-21 with enhanced in vivo therapeutic potency, Proc Natl Acad Sci U S A 117(51) (2020) 32370-32379. [CrossRef]
- Y.Y. Syed, Eteplirsen: First Global Approval, Drugs 76(17) (2016) 1699-1704. [CrossRef]
- B.T. Le, S. Paul, K. Jastrzebska, H. Langer, M.H. Caruthers, R.N. Veedu, Thiomorpholino oligonucleotides as a robust class of next generation platforms for alternate mRNA splicing, Proc Natl Acad Sci U S A 119(36) (2022) e2207956119. [CrossRef]
- V. MacLelland, M. Kravitz, A. Gupta, Therapeutic and diagnostic applications of antisense peptide nucleic acids, Mol Ther Nucleic Acids 35(1) (2024) 102086. [CrossRef]
- H. Asanuma, Y. Kamiya, H. Kashida, K. Murayama, Xeno nucleic acids (XNAs) having non-ribose scaffolds with unique supramolecular properties, Chem Commun (Camb) 58(25) (2022) 3993-4004. [CrossRef]
- K. Murayama, Y. Yamano, H. Asanuma, 8-Pyrenylvinyl Adenine Controls Reversible Duplex Formation between Serinol Nucleic Acid and RNA by [2 + 2] Photocycloaddition, J Am Chem Soc 141(24) (2019) 9485-9489. [CrossRef]
- T. Yoshida, T. Hagihara, Y. Uchida, Y. Horiuchi, K. Sasaki, T. Yamamoto, T. Yamashita, Y. Goda, Y. Saito, T. Yamaguchi, S. Obika, S. Yamamoto, T. Inoue, Introduction of sugar-modified nucleotides into CpG-containing antisense oligonucleotides inhibits TLR9 activation, Sci Rep 14(1) (2024) 11540. [CrossRef]
- S.T. Crooke, B.F. Baker, R.M. Crooke, X.H. Liang, Antisense technology: an overview and prospectus, Nat Rev Drug Discov 20(6) (2021) 427-453. [CrossRef]
- S.T. Crooke, B.F. Baker, J.L. Witztum, T.J. Kwoh, N.C. Pham, N. Salgado, B.W. McEvoy, W. Cheng, S.G. Hughes, S. Bhanot, R.S. Geary, The Effects of 2'-O-Methoxyethyl Containing Antisense Oligonucleotides on Platelets in Human Clinical Trials, Nucleic Acid Ther 27(3) (2017) 121-129. [CrossRef]
- H. Abou Assi, A.K. Rangadurai, H. Shi, B. Liu, M.C. Clay, K. Erharter, C. Kreutz, C.L. Holley, H.M. Al-Hashimi, 2'-O-Methylation can increase the abundance and lifetime of alternative RNA conformational states, Nucleic Acids Res 48(21) (2020) 12365-12379. [CrossRef]
- L. Sheng, F. Rigo, C.F. Bennett, A.R. Krainer, Y. Hua, Comparison of the efficacy of MOE and PMO modifications of systemic antisense oligonucleotides in a severe SMA mouse model, Nucleic Acids Res 48(6) (2020) 2853-2865. [CrossRef]
- Y. Masaki, Y. Iriyama, H. Nakajima, Y. Kuroda, T. Kanaki, S. Furukawa, M. Sekine, K. Seio, Application of 2'-O-(2-N-Methylcarbamoylethyl) Nucleotides in RNase H-Dependent Antisense Oligonucleotides, Nucleic Acid Ther 28(5) (2018) 307-311. [CrossRef]
- T. Yamaguchi, H. Komine, T. Sugiura, R. Kumagai, T. Yoshida, K. Sasaki, T. Nakayama, H. Kamada, T. Inoue, S. Obika, Cycloalkane Incorporation Into the 2',4'-Bridge of Locked Nucleic Acid: Enhancing Nuclease Stability, Reducing Phosphorothioate Modifications, and Lowering Hepatotoxicity in Antisense Oligonucleotides, JACS Au 5(10) (2025) 5111-5120. [CrossRef]
- P.H. Hagedorn, R. Persson, E.D. Funder, N. Albæk, S.L. Diemer, D.J. Hansen, M.R. Møller, N. Papargyri, H. Christiansen, B.R. Hansen, H.F. Hansen, M.A. Jensen, T. Koch, Locked nucleic acid: modality, diversity, and drug discovery, Drug Discov Today 23(1) (2018) 101-114. [CrossRef]
- N. Papargyri, M. Pontoppidan, M.R. Andersen, T. Koch, P.H. Hagedorn, Chemical Diversity of Locked Nucleic Acid-Modified Antisense Oligonucleotides Allows Optimization of Pharmaceutical Properties, Mol Ther Nucleic Acids 19 (2020) 706-717. [CrossRef]
- T. Matsubayashi, K. Yoshioka, S.S. Lei Mon, M. Katsuyama, C. Jia, T. Yamaguchi, R.I. Hara, T. Nagata, O. Nakagawa, S. Obika, T. Yokota, Favorable efficacy and reduced acute neurotoxicity by antisense oligonucleotides with 2',4'-BNA/LNA with 9-(aminoethoxy)phenoxazine, Mol Ther Nucleic Acids 35(2) (2024) 102161.
- U.S. Haque, T. Yokota, Enhancing Antisense Oligonucleotide-Based Therapeutic Delivery with DG9, a Versatile Cell-Penetrating Peptide, Cells 12(19) (2023). [CrossRef]
- Y. Nan, Y.J. Zhang, Antisense Phosphorodiamidate Morpholino Oligomers as Novel Antiviral Compounds, Front Microbiol 9 (2018) 750. [CrossRef]
- X. Sun, S. Setrerrahmane, C. Li, J. Hu, H. Xu, Nucleic acid drugs: recent progress and future perspectives, Signal Transduct Target Ther 9(1) (2024) 316. [CrossRef]
- A.J. Pollak, L. Zhao, T.A. Vickers, I.J. Huggins, X.H. Liang, S.T. Crooke, Insights into innate immune activation via PS-ASO-protein-TLR9 interactions, Nucleic Acids Res 50(14) (2022) 8107-8126. [CrossRef]
- J. He, F. Seela, Propynyl groups in duplex DNA: stability of base pairs incorporating 7-substituted 8-aza-7-deazapurines or 5-substituted pyrimidines, Nucleic Acids Res 30(24) (2002) 5485-96. [CrossRef]
- J.I. Gyi, D. Gao, G.L. Conn, J.O. Trent, T. Brown, A.N. Lane, The solution structure of a DNA*RNA duplex containing 5-propynyl U and C; comparison with 5-Me modifications, Nucleic Acids Res 31(10) (2003) 2683-93.
- A. Das, A. Ghosh, J. Kundu, M. Egli, M. Manoharan, S. Sinha, Synthesis and Biophysical Studies of High-Affinity Morpholino Oligomers Containing G-Clamp Analogs, J Org Chem 88(21) (2023) 15168-15175. [CrossRef]
- G. Fracchioni, S. Vailati, M. Grazioli, V. Pirota, Structural Unfolding of G-Quadruplexes: From Small Molecules to Antisense Strategies, Molecules 29(15) (2024). [CrossRef]
- L.P. Aiello, A.J. Brucker, S. Chang, E.T. Cunningham, Jr., D.J. D'Amico, H.W. Flynn, Jr., L.R. Grillone, S. Hutcherson, J.M. Liebmann, T.P. O'Brien, I.U. Scott, R.F. Spaide, C. Ta, M.T. Trese, Evolving guidelines for intravitreous injections, Retina 24(5 Suppl) (2004) S3-19. [CrossRef]
- J.M. Migliorati, S. Liu, A. Liu, A. Gogate, S. Nair, R. Bahal, T.P. Rasmussen, J.E. Manautou, X.B. Zhong, Absorption, Distribution, Metabolism, and Excretion of US Food and Drug Administration-Approved Antisense Oligonucleotide Drugs, Drug Metab Dispos 50(6) (2022) 888-897.
- D. Wu, Q. Chen, X. Chen, F. Han, Z. Chen, Y. Wang, The blood-brain barrier: structure, regulation, and drug delivery, Signal Transduct Target Ther 8(1) (2023) 217. [CrossRef]
- M. Monine, D. Norris, Y. Wang, I. Nestorov, A physiologically-based pharmacokinetic model to describe antisense oligonucleotide distribution after intrathecal administration, J Pharmacokinet Pharmacodyn 48(5) (2021) 639-654. [CrossRef]
- C.A. Chiriboga, K.J. Swoboda, B.T. Darras, S.T. Iannaccone, J. Montes, D.C. De Vivo, D.A. Norris, C.F. Bennett, K.M. Bishop, Results from a phase 1 study of nusinersen (ISIS-SMN(Rx)) in children with spinal muscular atrophy, Neurology 86(10) (2016) 890-7. [CrossRef]
- P. Anand, Y. Zhang, S. Patil, K. Kaur, Metabolic Stability and Targeted Delivery of Oligonucleotides: Advancing RNA Therapeutics Beyond The Liver, J Med Chem 68(7) (2025) 6870-6896. [CrossRef]
- M.F. Yuen, S.G. Lim, R. Plesniak, K. Tsuji, H.L.A. Janssen, C. Pojoga, A. Gadano, C.P. Popescu, T. Stepanova, T. Asselah, G. Diaconescu, H.J. Yim, J. Heo, E. Janczewska, A. Wong, N. Idriz, M. Imamura, G. Rizzardini, K. Takaguchi, P. Andreone, M. Arbune, J. Hou, S.J. Park, A. Vata, J. Cremer, R. Elston, T. Lukić, G. Quinn, L. Maynard, S. Kendrick, H. Plein, F. Campbell, M. Paff, D. Theodore, Efficacy and Safety of Bepirovirsen in Chronic Hepatitis B Infection, N Engl J Med 387(21) (2022) 1957-1968. [CrossRef]
- M.F. Yuen, J. Heo, J.W. Jang, J.H. Yoon, Y.O. Kweon, S.J. Park, Y. Tami, S. You, P. Yates, Y. Tao, J. Cremer, F. Campbell, R. Elston, D. Theodore, M. Paff, C.F. Bennett, T.J. Kwoh, Safety, tolerability and antiviral activity of the antisense oligonucleotide bepirovirsen in patients with chronic hepatitis B: a phase 2 randomized controlled trial, Nat Med 27(10) (2021) 1725-1734. [CrossRef]
- A. Vaillant, Bepirovirsen/GSK3389404: Antisense or TLR9 agonists?, J Hepatol 78(3) (2023) e107-e108. [CrossRef]
- M.F. Yuen, J. Heo, H. Kumada, F. Suzuki, Y. Suzuki, Q. Xie, J. Jia, Y. Karino, J. Hou, K. Chayama, M. Imamura, J.Y. Lao-Tan, S.G. Lim, Y. Tanaka, W. Xie, J.H. Yoon, Z. Duan, M. Kurosaki, S.J. Park, M.E. Labio, R. Kumar, Y.O. Kweon, H.J. Yim, Y. Tao, J. Cremer, R. Elston, M. Davies, S. Baptiste-Brown, K. Han, F.M. Campbell, M. Paff, D. Theodore, Phase IIa, randomised, double-blind study of GSK3389404 in patients with chronic hepatitis B on stable nucleos(t)ide therapy, J Hepatol 77(4) (2022) 967-977. [CrossRef]
- R.W. Hui, L.Y. Mak, J. Fung, W.K. Seto, M.F. Yuen, Prospect of emerging treatments for hepatitis B virus functional cure, Clin Mol Hepatol 31(Suppl) (2025) S165-181. [CrossRef]
- R.A. Goodnow, Reality check: lipid-oligonucleotide conjugates for therapeutic applications, Expert Opin Drug Discov 18(2) (2023) 129-134. [CrossRef]
- S. Shahnoor, I.F. Raza, M. Rashid, H. Panhwar, I. Fatima, S. Gul, K. Nadeem, S. Khan, M. Mahmmoud Fadelallah Eljack, FDA approval of imetelstat: a new era in the treatment of lower-risk myelodysplastic syndrome, Ann Med Surg (Lond) 87(12) (2025) 8385-8390. [CrossRef]
- U. Platzbecker, V. Santini, P. Fenaux, M.A. Sekeres, M.R. Savona, Y.F. Madanat, M. Díez-Campelo, D. Valcárcel, T. Illmer, A. Jonášová, P. Bělohlávková, L.J. Sherman, T. Berry, S. Dougherty, S. Shah, Q. Xia, L. Sun, Y. Wan, F. Huang, A. Ikin, S. Navada, F. Feller, R.S. Komrokji, A.M. Zeidan, Imetelstat in patients with lower-risk myelodysplastic syndromes who have relapsed or are refractory to erythropoiesis-stimulating agents (IMerge): a multinational, randomised, double-blind, placebo-controlled, phase 3 trial, Lancet 403(10423) (2024) 249-260. [CrossRef]
- T.P. Prakash, A.E. Mullick, R.G. Lee, J. Yu, S.T. Yeh, A. Low, A.E. Chappell, M.E. Østergaard, S. Murray, H.J. Gaus, E.E. Swayze, P.P. Seth, Fatty acid conjugation enhances potency of antisense oligonucleotides in muscle, Nucleic Acids Res 47(12) (2019) 6029-6044. [CrossRef]
- A.A. Balachandran, B.H. Poudel, K. Rahimizadeh, A. Chikkanna, R.N. Veedu, Enhancing the intracellular delivery of antisense oligonucleotides (ASO) : a comparative study of aptamer, vitamin E, and cholesterol ASO conjugates, RSC Adv 15(51) (2025) 43727-43736. [CrossRef]
- P. Mangla, Q. Vicentini, A. Biscans, Therapeutic Oligonucleotides: An Outlook on Chemical Strategies to Improve Endosomal Trafficking, Cells 12(18) (2023). [CrossRef]
- B. Malecova, R.S. Burke, M. Cochran, M.D. Hood, R. Johns, P.R. Kovach, V.R. Doppalapudi, G. Erdogan, J.D. Arias, B. Darimont, C.D. Miller, H. Huang, A. Geall, H.S. Younis, A.A. Levin, Targeted tissue delivery of RNA therapeutics using antibody-oligonucleotide conjugates (AOCs), Nucleic Acids Res 51(12) (2023) 5901-5910. [CrossRef]
- M. Cochran, D. Arias, R. Burke, D. Chu, G. Erdogan, M. Hood, P. Kovach, H.W. Kwon, Y. Chen, M. Moon, C.D. Miller, H. Huang, A. Levin, V.R. Doppalapudi, Structure-Activity Relationship of Antibody-Oligonucleotide Conjugates: Evaluating Bioconjugation Strategies for Antibody-siRNA Conjugates for Drug Development, J Med Chem 67(17) (2024) 14852-14867. [CrossRef]
- L.V. Gushchina, T.A. Vetter, E.C. Frair, A.J. Bradley, K.M. Grounds, J.W. Lay, N. Huang, A. Suhaiba, F.J. Schnell, G. Hanson, T.R. Simmons, N. Wein, K.M. Flanigan, Systemic PPMO-mediated dystrophin expression in the Dup2 mouse model of Duchenne muscular dystrophy, Mol Ther Nucleic Acids 30 (2022) 479-492. [CrossRef]
- W. Yang, C. Ran, X. Lian, Z. Wang, Z. Du, T. Bing, Y. Zhang, W. Tan, Aptamer-based targeted drug delivery and disease therapy in preclinical and clinical applications, Adv Drug Deliv Rev 226 (2025) 115680. [CrossRef]
- F. Millozzi, P. Milán-Rois, A. Sett, G. Delli Carpini, M. De Bardi, M. Gisbert-Garzarán, M. Sandonà, C. Rodríguez-Díaz, M. Martínez-Mingo, I. Pardo, F. Esposito, M.T. Viscomi, M. Bouché, O. Parolini, V. Saccone, J.J. Toulmé, Á. Somoza, D. Palacios, Aptamer-conjugated gold nanoparticles enable oligonucleotide delivery into muscle stem cells to promote regeneration of dystrophic muscles, Nat Commun 16(1) (2025) 577. [CrossRef]
- M. Mehta, T.A. Bui, X. Yang, Y. Aksoy, E.M. Goldys, W. Deng, Lipid-Based Nanoparticles for Drug/Gene Delivery: An Overview of the Production Techniques and Difficulties Encountered in Their Industrial Development, ACS Mater Au 3(6) (2023) 600-619. [CrossRef]
- P.R. Cullis, P.L. Felgner, The 60-year evolution of lipid nanoparticles for nucleic acid delivery, Nat Rev Drug Discov 23(9) (2024) 709-722. [CrossRef]
- R. Jeitler, C. Glader, G. König, J. Kaplan, C. Tetyczka, J. Remmelgas, M. Mußbacher, E. Fröhlich, E. Roblegg, On the Structure, Stability, and Cell Uptake of Nanostructured Lipid Carriers for Drug Delivery, Mol Pharm 21(7) (2024) 3674-3683. [CrossRef]
- M.L. Borrajo, A. Quijano, P. Lapuhs, A.I. Rodriguez-Perez, S. Anthiya, J.L. Labandeira-Garcia, R. Valenzuela, M.J. Alonso, Ionizable nanoemulsions for RNA delivery into the central nervous system - importance of diffusivity, J Control Release 372 (2024) 295-303. [CrossRef]
- X. Cai, R. Dou, C. Guo, J. Tang, X. Li, J. Chen, J. Zhang, Cationic Polymers as Transfection Reagents for Nucleic Acid Delivery, Pharmaceutics 15(5) (2023). [CrossRef]
- H. Takakusa, N. Iwazaki, M. Nishikawa, T. Yoshida, S. Obika, T. Inoue, Drug Metabolism and Pharmacokinetics of Antisense Oligonucleotide Therapeutics: Typical Profiles, Evaluation Approaches, and Points to Consider Compared with Small Molecule Drugs, Nucleic Acid Therapeutics 33(2) (2023) 83-94. [CrossRef]
- D.C. Luther, R. Huang, T. Jeon, X. Zhang, Y.W. Lee, H. Nagaraj, V.M. Rotello, Delivery of drugs, proteins, and nucleic acids using inorganic nanoparticles, Adv Drug Deliv Rev 156 (2020) 188-213. [CrossRef]
- Y. Liu, M. Zhao, M. Zhang, B. Yang, Y.K. Qi, Q. Fu, Mesoporous silica nanoparticle-based nanomedicine: Preparation, functional modification, and theranostic applications, Mater Today Bio 34 (2025) 102223. [CrossRef]
- A.R. Sharma, Y.H. Lee, A. Bat-Ulzii, M. Bhattacharya, C. Chakraborty, S.S. Lee, Recent advances of metal-based nanoparticles in nucleic acid delivery for therapeutic applications, J Nanobiotechnology 20(1) (2022) 501. [CrossRef]
- C.R. Garza-Cardenas, A. Leon-Buitimea, A.A. Siller-Ceniceros, J.R. Morones-Ramirez, Antisense Oligonucleotide-Capped Gold Nanoparticles as a Potential Strategy for Tackling Antimicrobial Resistance, Microbiology Research 16(3) (2025) 70. [CrossRef]
- R. Lapusan, R. Borlan, M. Focsan, Advancing MRI with magnetic nanoparticles: a comprehensive review of translational research and clinical trials, Nanoscale Adv 6(9) (2024) 2234-2259. [CrossRef]
- M. Liu, B. Chu, R. Sun, J. Ding, H. Ye, Y. Yang, Y. Wu, H. Shi, B. Song, Y. He, H. Wang, J. Hong, Antisense Oligonucleotides Selectively Enter Human-Derived Antibiotic-Resistant Bacteria through Bacterial-Specific ATP-Binding Cassette Sugar Transporter, Adv Mater 35(28) (2023) e2300477. [CrossRef]
- G. Xu, J. Jin, Z. Fu, G. Wang, X. Lei, J. Xu, J. Wang, Extracellular vesicle-based drug overview: research landscape, quality control and nonclinical evaluation strategies, Signal Transduct Target Ther 10(1) (2025) 255. [CrossRef]
- M. Zhang, S. Hu, L. Liu, P. Dang, Y. Liu, Z. Sun, B. Qiao, C. Wang, Engineered exosomes from different sources for cancer-targeted therapy, Signal Transduct Target Ther 8(1) (2023) 124. [CrossRef]
- S. Kamerkar, C. Leng, O. Burenkova, S.C. Jang, C. McCoy, K. Zhang, K. Dooley, S. Kasera, T. Zi, S. Sisó, W. Dahlberg, C.L. Sia, S. Patel, K. Schmidt, K. Economides, T. Soos, D. Burzyn, S. Sathyanarayanan, Exosome-mediated genetic reprogramming of tumor-associated macrophages by exoASO-STAT6 leads to potent monotherapy antitumor activity, Sci Adv 8(7) (2022) eabj7002. [CrossRef]
- L. Liu, D. Pan, S. Chen, M.V. Martikainen, A. Kårlund, J. Ke, H. Pulkkinen, H. Ruhanen, M. Roponen, R. Käkelä, W. Xu, J. Wang, V.P. Lehto, Systematic design of cell membrane coating to improve tumor targeting of nanoparticles, Nat Commun 13(1) (2022) 6181. [CrossRef]
- A. Gogate, J. Belcourt, M. Shah, A.Z. Wang, A. Frankel, H. Kolmel, M. Chalon, P. Stephen, A. Kolli, S.M. Tawfik, J. Jin, R. Bahal, T.P. Rasmussen, J.E. Manautou, X.B. Zhong, Targeting the Liver with Nucleic Acid Therapeutics for the Treatment of Systemic Diseases of Liver Origin, Pharmacol Rev 76(1) (2023) 49-89. [CrossRef]
- J.L. Witztum, D. Gaudet, S.D. Freedman, V.J. Alexander, A. Digenio, K.R. Williams, Q. Yang, S.G. Hughes, R.S. Geary, M. Arca, E.S.G. Stroes, J. Bergeron, H. Soran, F. Civeira, L. Hemphill, S. Tsimikas, D.J. Blom, L. O'Dea, E. Bruckert, Volanesorsen and Triglyceride Levels in Familial Chylomicronemia Syndrome, N Engl J Med 381(6) (2019) 531-542. [CrossRef]
- L. De Michieli, A. Lupi, G. Sinigiani, A. Tietto, A. Salvalaggio, A. Branca, S. Da Pozzo, S. Rizzo, D. Cecchin, M. Perazzolo Marra, T. Berno, D. Corrado, C. Briani, A. Cipriani, Pharmacological Management of Transthyretin Amyloid Cardiomyopathy: Where We Are and Where We Are Going, J Clin Med 14(10) (2025). [CrossRef]
- L. Xu, I. Irony, W.W. Bryan, B. Dunn, Development of gene therapies-lessons from nusinersen, Gene Ther 24(9) (2017) 527-528. [CrossRef]
- A. McGuigan, H.A. Blair, Tofersen: A Review in Amyotrophic Lateral Sclerosis Associated with SOD1 Mutations, CNS Drugs 39(9) (2025) 903-912. [CrossRef]
- S.J. Keam, Imetelstat: First Approval, Drugs 84(9) (2024) 1149-1155. [CrossRef]
- Y. Abaza, A.E. DeZern, Imetelstat: a new addition to the therapeutic landscape of lower-risk MDS, Blood 145(5) (2025) 469-474. [CrossRef]
- M.A. Riedl, R. Tachdjian, W.R. Lumry, T. Craig, G. Karakaya, A. Gelincik, M. Stobiecki, J.S. Jacobs, N.M. Gokmen, A. Reshef, M.M. Gompels, M.E. Manning, L. Bordone, K.B. Newman, S. Treadwell, S. Wang, A. Yarlas, D.M. Cohn, Efficacy and Safety of Donidalorsen for Hereditary Angioedema, N Engl J Med 391(1) (2024) 21-31. [CrossRef]
- B.A. Bergmark, N.A. Marston, C.R. Bramson, M. Curto, V. Ramos, A. Jevne, J.F. Kuder, J.G. Park, S.A. Murphy, S. Verma, W. Wojakowski, S.G. Terra, M.S. Sabatine, S.D. Wiviott, Effect of Vupanorsen on Non-High-Density Lipoprotein Cholesterol Levels in Statin-Treated Patients With Elevated Cholesterol: TRANSLATE-TIMI 70, Circulation 145(18) (2022) 1377-1386. [CrossRef]
- K. Chwalenia, M.J.A. Wood, T.C. Roberts, Progress and prospects in antisense oligonucleotide-mediated exon skipping therapies for Duchenne muscular dystrophy, J Muscle Res Cell Motil 46(4) (2025) 293-300. [CrossRef]
- Food and Drug Administration (FDA), Clinical Pharmacology Considerations for the Development of Oligonucleotide Therapeutics, 2026-01-30. https://www.fda.gov/regulatory-information/search-fda-guidance-documents/clinical-pharmacology-considerations-development-oligonucleotide-therapeutics.
- T.B. Emran, A. Shahriar, A.R. Mahmud, T. Rahman, M.H. Abir, M.F. Siddiquee, H. Ahmed, N. Rahman, F. Nainu, E. Wahyudin, S. Mitra, K. Dhama, M.M. Habiballah, S. Haque, A. Islam, M.M. Hassan, Multidrug Resistance in Cancer: Understanding Molecular Mechanisms, Immunoprevention and Therapeutic Approaches, Front Oncol 12 (2022) 891652. [CrossRef]
- M. Nikanjam, S. Kato, T. Allen, J.K. Sicklick, R. Kurzrock, Novel clinical trial designs emerging from the molecular reclassification of cancer, CA Cancer J Clin 75(3) (2025) 243-267. [CrossRef]
- K.N. Chi, C.S. Higano, B. Blumenstein, J.M. Ferrero, J. Reeves, S. Feyerabend, G. Gravis, A.S. Merseburger, A. Stenzl, A.M. Bergman, S.D. Mukherjee, P. Zalewski, F. Saad, C. Jacobs, M. Gleave, J.S. de Bono, Custirsen in combination with docetaxel and prednisone for patients with metastatic castration-resistant prostate cancer (SYNERGY trial): a phase 3, multicentre, open-label, randomised trial, Lancet Oncol 18(4) (2017) 473-485. [CrossRef]
- T.M. Beer, S.J. Hotte, F. Saad, B. Alekseev, V. Matveev, A. Fléchon, G. Gravis, F. Joly, K.N. Chi, Z. Malik, B. Blumenstein, P.S. Stewart, C.A. Jacobs, K. Fizazi, Custirsen (OGX-011) combined with cabazitaxel and prednisone versus cabazitaxel and prednisone alone in patients with metastatic castration-resistant prostate cancer previously treated with docetaxel (AFFINITY): a randomised, open-label, international, phase 3 trial, Lancet Oncol 18(11) (2017) 1532-1542. [CrossRef]
- Clinicaltrials.gov, Study of SRP-4045 (Casimersen) and SRP-4053 (Golodirsen) in Participants With Duchenne Muscular Dystrophy (DMD) (ESSENCE), 2025-11-18. https://clinicaltrials.gov/study/NCT02500381.
- Parent Project Muscular Dystrophy, Sarepta Announces Completion of ESSENCE Trial for Exon 45 & 53 Skipping Therapies, 2026-01-30. https://www.parentprojectmd.org/sarepta-announces-completion-of-essence-trial-for-exon-45-53-skipping-therapies.
- Clinicaltrials.gov, A Study to Evaluate Efficacy, Safety, Tolerability and Exposure After a Repeat-dose of Sepofarsen (QR-110) in LCA10 (ILLUMINATE) (ILLUMINATE), 2022-03-17. https://clinicaltrials.gov/study/NCT03913143.
- S.R. Russell, A.V. Drack, A.V. Cideciyan, S.G. Jacobson, B.P. Leroy, C. Van Cauwenbergh, A.C. Ho, A.V. Dumitrescu, I.C. Han, M. Martin, W.L. Pfeifer, E.H. Sohn, J. Walshire, A.V. Garafalo, A.K. Krishnan, C.A. Powers, A. Sumaroka, A.J. Roman, E. Vanhonsebrouck, E. Jones, F. Nerinckx, J. De Zaeytijd, R.W.J. Collin, C. Hoyng, P. Adamson, M.E. Cheetham, M.R. Schwartz, W. den Hollander, F. Asmus, G. Platenburg, D. Rodman, A. Girach, Intravitreal antisense oligonucleotide sepofarsen in Leber congenital amaurosis type 10: a phase 1b/2 trial, Nat Med 28(5) (2022) 1014-1021. [CrossRef]
- J. Saade, T.A. Mestre, Huntington's Disease: Latest Frontiers in Therapeutics, Curr Neurol Neurosci Rep 24(8) (2024) 255-264. [CrossRef]
- P. McColgan, A. Thobhani, L. Boak, S.A. Schobel, A. Nicotra, G. Palermo, D. Trundell, J. Zhou, V. Schlegel, P. Sanwald Ducray, D.J. Hawellek, J. Dorn, C. Simillion, M. Lindemann, V. Wheelock, A. Durr, K.E. Anderson, J.D. Long, E.J. Wild, G.B. Landwehrmeyer, B.R. Leavitt, S.J. Tabrizi, R. Doody, Tominersen in Adults with Manifest Huntington's Disease, N Engl J Med 389(23) (2023) 2203-2205. [CrossRef]
- J.Y. Yao, T. Liu, X.R. Hu, H. Sheng, Z.H. Chen, H.Y. Zhao, X.J. Li, Y. Wang, L. Hao, An insight into allele-selective approaches to lowering mutant huntingtin protein for Huntington's disease treatment, Biomed Pharmacother 180 (2024) 117557. [CrossRef]
- European Medicines Agency(EMA), Vitravene, 2002-07-08. https://www.ema.europa.eu/en/medicines/human/EPAR/vitravene.
- Clinicaltrials.gov, Assessing the Impact of Lipoprotein (a) Lowering With Pelacarsen (TQJ230) on Major Cardiovascular Events in Patients With CVD (Lp(a)HORIZON), 2025-12-31. https://clinicaltrials.gov/study/NCT04023552.
- ClinicalTrials.gov, Phase 3 Efficacy and Safety Study of GTX-102 in Pediatric Subjects With Angelman Syndrome (AS) (Aspire), 2025-11-06. https://clinicaltrials.gov/study/NCT06617429.
- ClinicalTrials.gov, Study of Bepirovirsen in Nucleos(t)Ide Analogue-treated Participants With Chronic Hepatitis B (B-Well 2) (B-Well 2), 2025-12-12. https://clinicaltrials.gov/study/NCT05630820.
- F. Jaschinski, T. Rothhammer, P. Jachimczak, C. Seitz, A. Schneider, K.H. Schlingensiepen, The antisense oligonucleotide trabedersen (AP 12009) for the targeted inhibition of TGF-β2, Curr Pharm Biotechnol 12(12) (2011) 2203-13. [CrossRef]
- S. Mariathasan, S.J. Turley, D. Nickles, A. Castiglioni, K. Yuen, Y. Wang, E.E. Kadel, III, H. Koeppen, J.L. Astarita, R. Cubas, S. Jhunjhunwala, R. Banchereau, Y. Yang, Y. Guan, C. Chalouni, J. Ziai, Y. Şenbabaoğlu, S. Santoro, D. Sheinson, J. Hung, J.M. Giltnane, A.A. Pierce, K. Mesh, S. Lianoglou, J. Riegler, R.A.D. Carano, P. Eriksson, M. Höglund, L. Somarriba, D.L. Halligan, M.S. van der Heijden, Y. Loriot, J.E. Rosenberg, L. Fong, I. Mellman, D.S. Chen, M. Green, C. Derleth, G.D. Fine, P.S. Hegde, R. Bourgon, T. Powles, TGFβ attenuates tumour response to PD-L1 blockade by contributing to exclusion of T cells, Nature 554(7693) (2018) 544-548. [CrossRef]
- ClinicalTrials.gov,, Trabedersen (OT-101) With Pembrolizumab for Newly Diagnosed Advanced NSCLC and Positive PD-L1, 2025-07-24. https://clinicaltrials.gov/study/NCT06579196.
- M. Li, H. An, J. Zhang, W. Li, C. Yu, L. Wang, Advances in the pharmaceutical development of antibody-oligonucleotide conjugates, Eur J Pharm Sci 215 (2025) 107292. [CrossRef]
- O. Kovecses, F.E. Mercier, M. McKeague, Nucleic acid therapeutics as differentiation agents for myeloid leukemias, Leukemia 38(7) (2024) 1441-1454. [CrossRef]
- V. Bhati, S. Prasad, A. Kabra, RNA-based therapies for neurodegenerative disease: Targeting molecular mechanisms for disease modification, Mol Cell Neurosci 133 (2025) 104010. [CrossRef]
- A. Bruch, A.A. Kelani, M.G. Blango, RNA-based therapeutics to treat human fungal infections, Trends Microbiol 30(5) (2022) 411-420. [CrossRef]
- D. Araújo, D. Mil-Homens, M. Henriques, S. Silva, Anti-EFG1 2'-OMethylRNA oligomer inhibits Candida albicans filamentation and attenuates the candidiasis in Galleria mellonella, Mol Ther Nucleic Acids 27 (2022) 517-523. [CrossRef]
- A. Barbosa, D. Araújo, M. Henriques, S. Silva, The combined application of the anti-RAS1 and anti-RIM101 2'-OMethylRNA oligomers enhances Candida albicans filamentation control, Med Mycol 59(10) (2021) 1024-1031.
- J.Y. Chung, Y.K. Hong, E. Jeon, S. Yang, A. Park, R. Weissleder, Y.P. Chong, H.J. Chung, Effective treatment of systemic candidiasis by synergistic targeting of cell wall synthesis, Nat Commun 16(1) (2025) 5532. [CrossRef]
- P.R. Carstens, T. Yokota, From Genomic Diagnosis to Personalized RNA Medicine: Advances in Next-Generation Sequencing and N-of-1 Antisense Oligonucleotide Therapies for Rare Genetic Diseases, Preprints, Preprints, 2025. [CrossRef]
- H. Wilton-Clark, E. Yan, T. Yokota, Milasen: The Emerging Era of Patient-Customized N-of-1 Antisense Oligonucleotides as Therapeutic Agents for Genetic Diseases, Methods Mol Biol 2964 (2025) 85-93.
- A. Aartsma-Rus, A. Garanto, W. van Roon-Mom, E.M. McConnell, V. Suslovitch, W.X. Yan, J.K. Watts, T.W. Yu, Consensus Guidelines for the Design and In Vitro Preclinical Efficacy Testing N-of-1 Exon Skipping Antisense Oligonucleotides, Nucleic Acid Ther 33(1) (2023) 17-25. [CrossRef]
- Y.F. Wu, J.A. Chen, Y.J. Jong, Treating neuromuscular diseases: unveiling gene therapy breakthroughs and pioneering future applications, J Biomed Sci 32(1) (2025) 30. [CrossRef]
- K.D. Kernohan, K.M. Boycott, The expanding diagnostic toolbox for rare genetic diseases, Nature Reviews Genetics 25(6) (2024) 401-415. [CrossRef]
- B.J. Booth, S. Nourreddine, D. Katrekar, Y. Savva, D. Bose, T.J. Long, D.J. Huss, P. Mali, RNA editing: Expanding the potential of RNA therapeutics, Mol Ther 31(6) (2023) 1533-1549. [CrossRef]
Figure 1.
Timeline of antisense oligonucleotide (ASO) technology development. This timeline delineates the three-stage evolutionary trajectory of ASOs technology: Inception and Preliminary Validation (1978–1990s), marked by the conceptualization of ASOs and early chemical modifications (e.g., phosphorothioate [PS]) leading to the first FDA-approved ASO (Fomivirsen); Setbacks and Technological Reshaping (2000s–2015), characterized by clinical trial challenges that drove advancements in second-generation chemistries (e.g., 2′-O-methoxyethyl [2′-MOE]) and targeted delivery (e.g., N-acetylgalactosamine [GalNAc] conjugation); and Clinical Explosion and the Golden Age (2016–present), defined by transformative approvals (e.g., Nusinersen for spinal muscular atrophy) and the maturation of ASOs as a versatile therapeutic platform. The figure was created with BioRender.com. PS: phosphorothioate; PMO: phosphorodiamidate morpholino oligomer; PNA: peptide nucleic acid; 2′-MOE: 2′-O-methoxyethyl; LNA: locked nucleic acid.
Figure 1.
Timeline of antisense oligonucleotide (ASO) technology development. This timeline delineates the three-stage evolutionary trajectory of ASOs technology: Inception and Preliminary Validation (1978–1990s), marked by the conceptualization of ASOs and early chemical modifications (e.g., phosphorothioate [PS]) leading to the first FDA-approved ASO (Fomivirsen); Setbacks and Technological Reshaping (2000s–2015), characterized by clinical trial challenges that drove advancements in second-generation chemistries (e.g., 2′-O-methoxyethyl [2′-MOE]) and targeted delivery (e.g., N-acetylgalactosamine [GalNAc] conjugation); and Clinical Explosion and the Golden Age (2016–present), defined by transformative approvals (e.g., Nusinersen for spinal muscular atrophy) and the maturation of ASOs as a versatile therapeutic platform. The figure was created with BioRender.com. PS: phosphorothioate; PMO: phosphorodiamidate morpholino oligomer; PNA: peptide nucleic acid; 2′-MOE: 2′-O-methoxyethyl; LNA: locked nucleic acid.
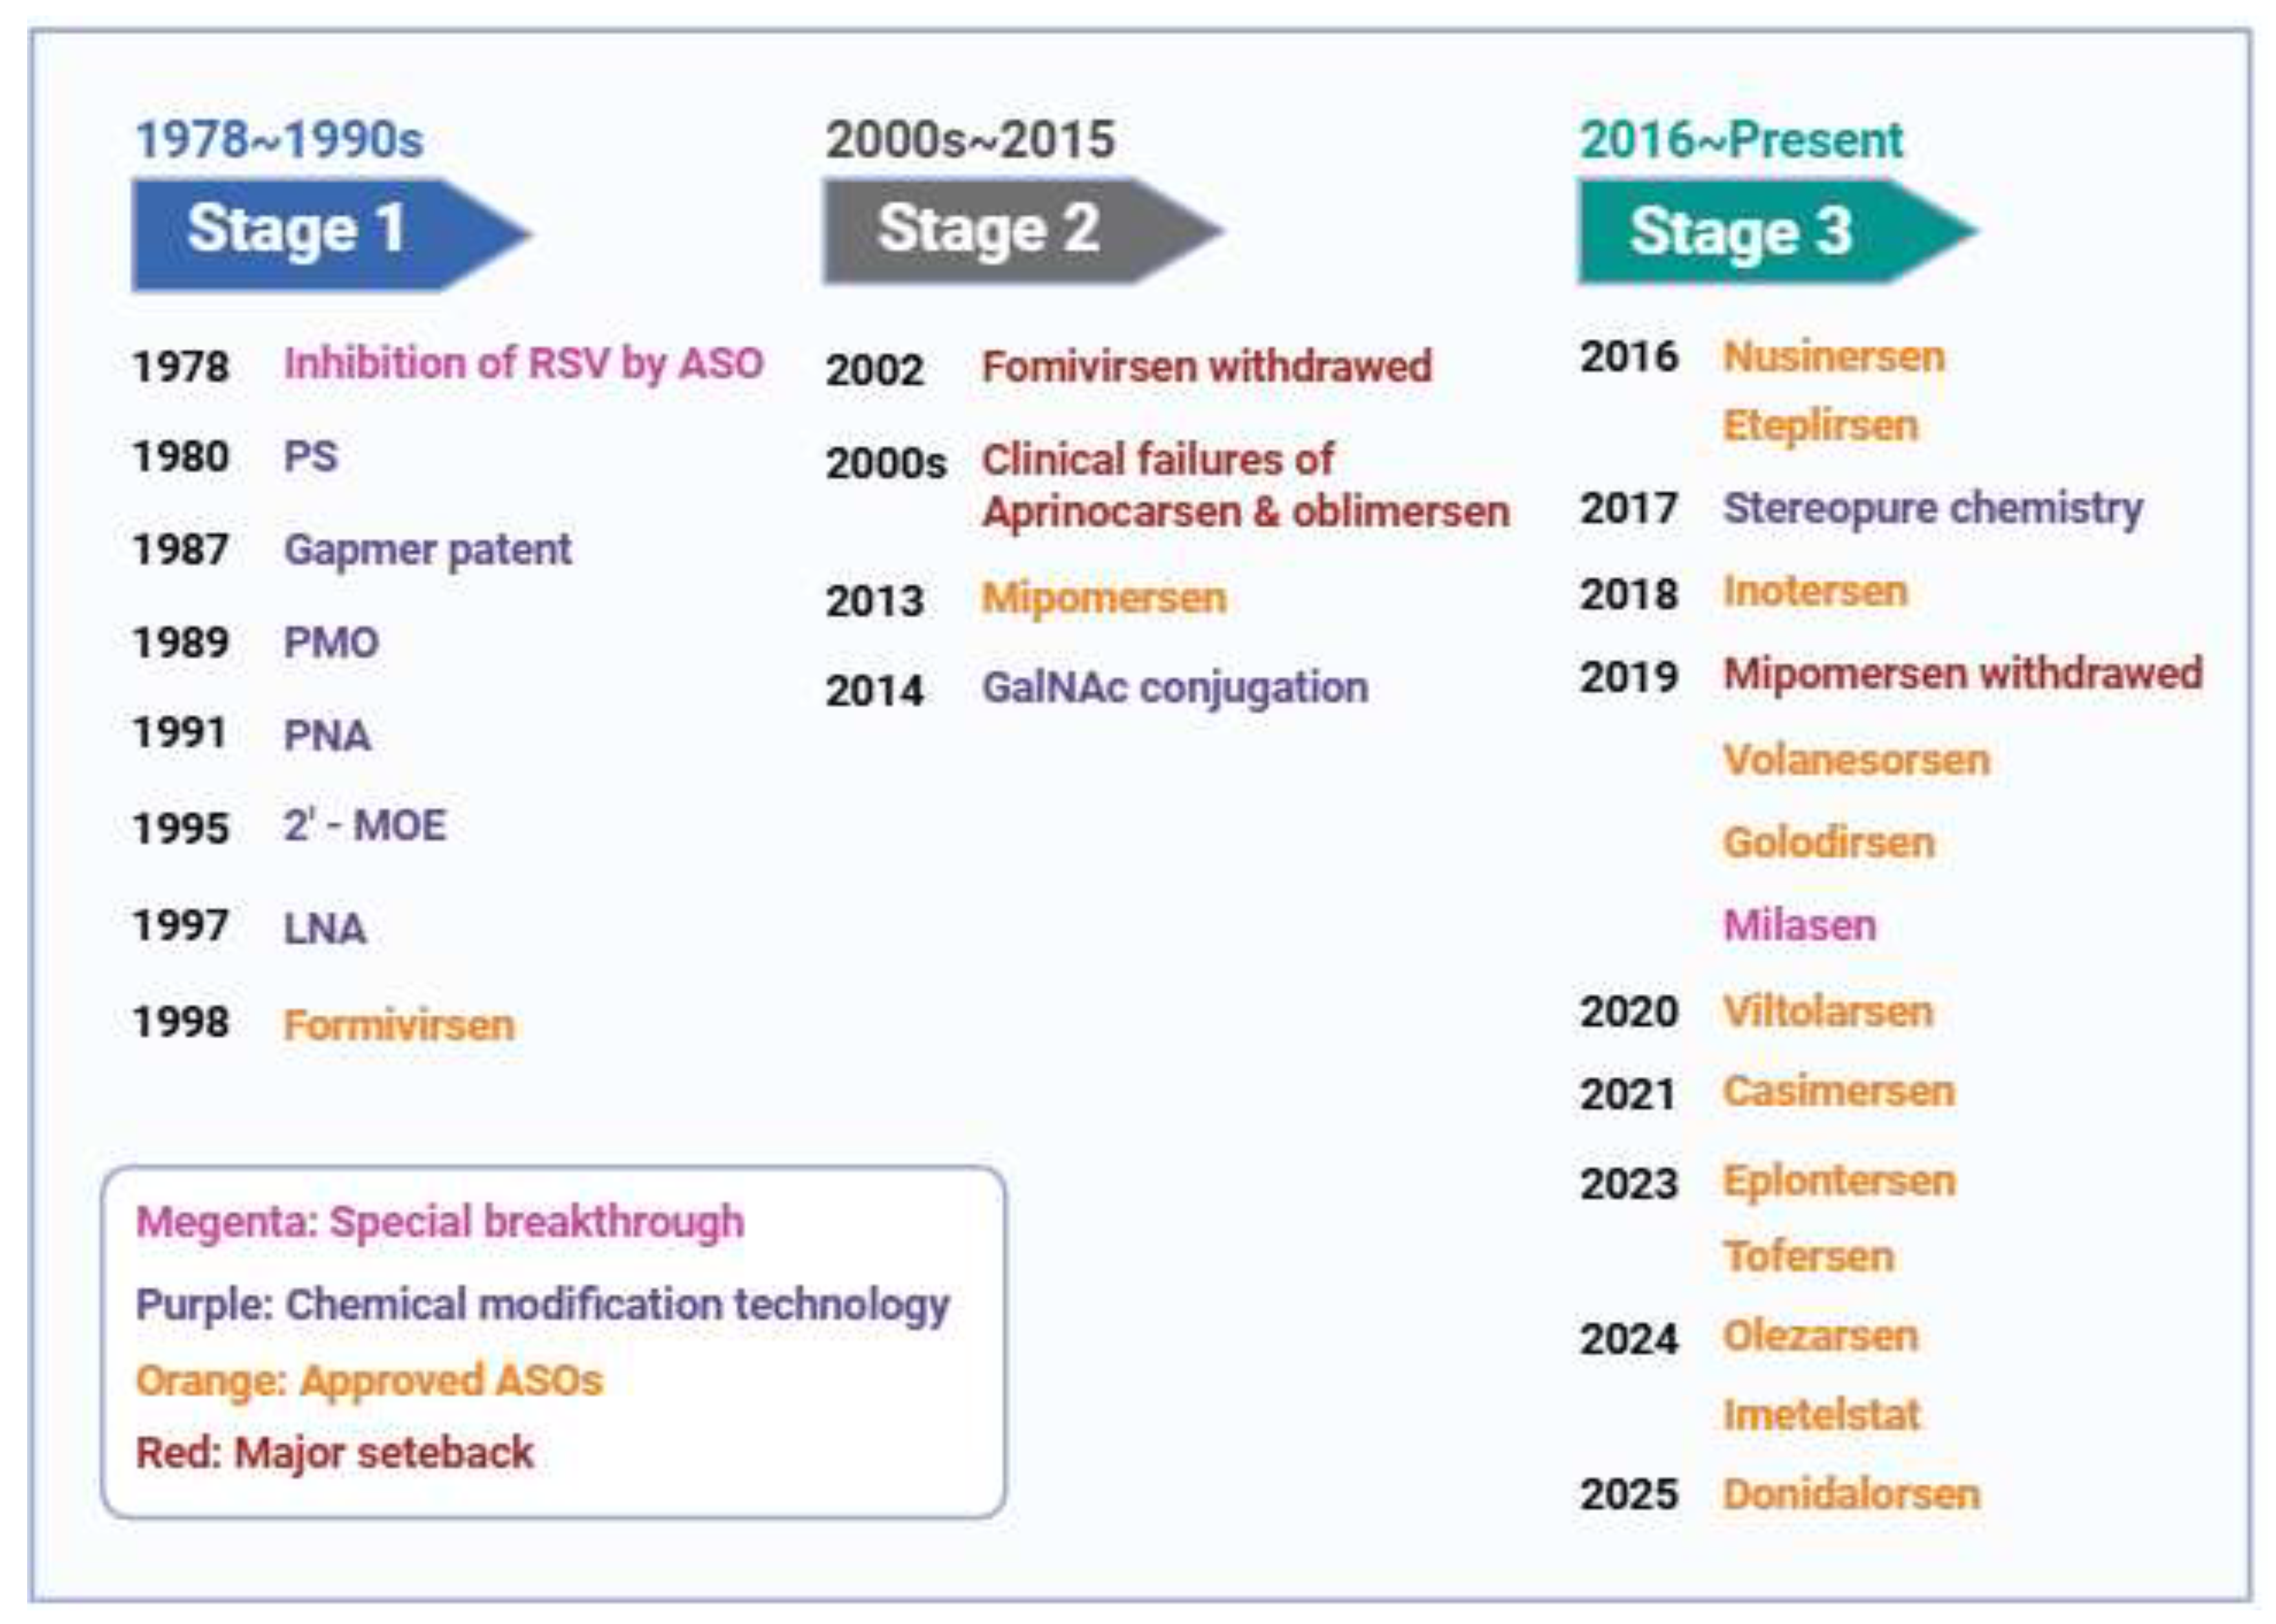
Figure 2.
Mechanism of actionof antisense oligonucleotides (ASOs). ASOs are internalized into target cells through endocytosis, traverse the endocytic pathway, undergo endosomal escape to reach the cytoplasm or nucleus. They modulate gene expression through two core mechanisms: (1) nuclease-mediated degradation, wherein ASO-target RNA heteroduplexes recruit RNase H1 to catalyze site-specific cleavage of pathogenic transcripts; and (2) steric blockade, which inhibits interactions between RNA and regulatory molecules (e.g., spliceosomes, ribosomes). Specific modes of action include RNase H1-mediated mRNA degradation, steric blockade-modulated alternative splicing (e.g., exon skipping to restore reading frames in dystrophin deficiency), and steric blockade-suppressed translation (e.g., binding to 5′ untranslated regions to inhibit initiation). The figure was created with BioRender.com.
Figure 2.
Mechanism of actionof antisense oligonucleotides (ASOs). ASOs are internalized into target cells through endocytosis, traverse the endocytic pathway, undergo endosomal escape to reach the cytoplasm or nucleus. They modulate gene expression through two core mechanisms: (1) nuclease-mediated degradation, wherein ASO-target RNA heteroduplexes recruit RNase H1 to catalyze site-specific cleavage of pathogenic transcripts; and (2) steric blockade, which inhibits interactions between RNA and regulatory molecules (e.g., spliceosomes, ribosomes). Specific modes of action include RNase H1-mediated mRNA degradation, steric blockade-modulated alternative splicing (e.g., exon skipping to restore reading frames in dystrophin deficiency), and steric blockade-suppressed translation (e.g., binding to 5′ untranslated regions to inhibit initiation). The figure was created with BioRender.com.
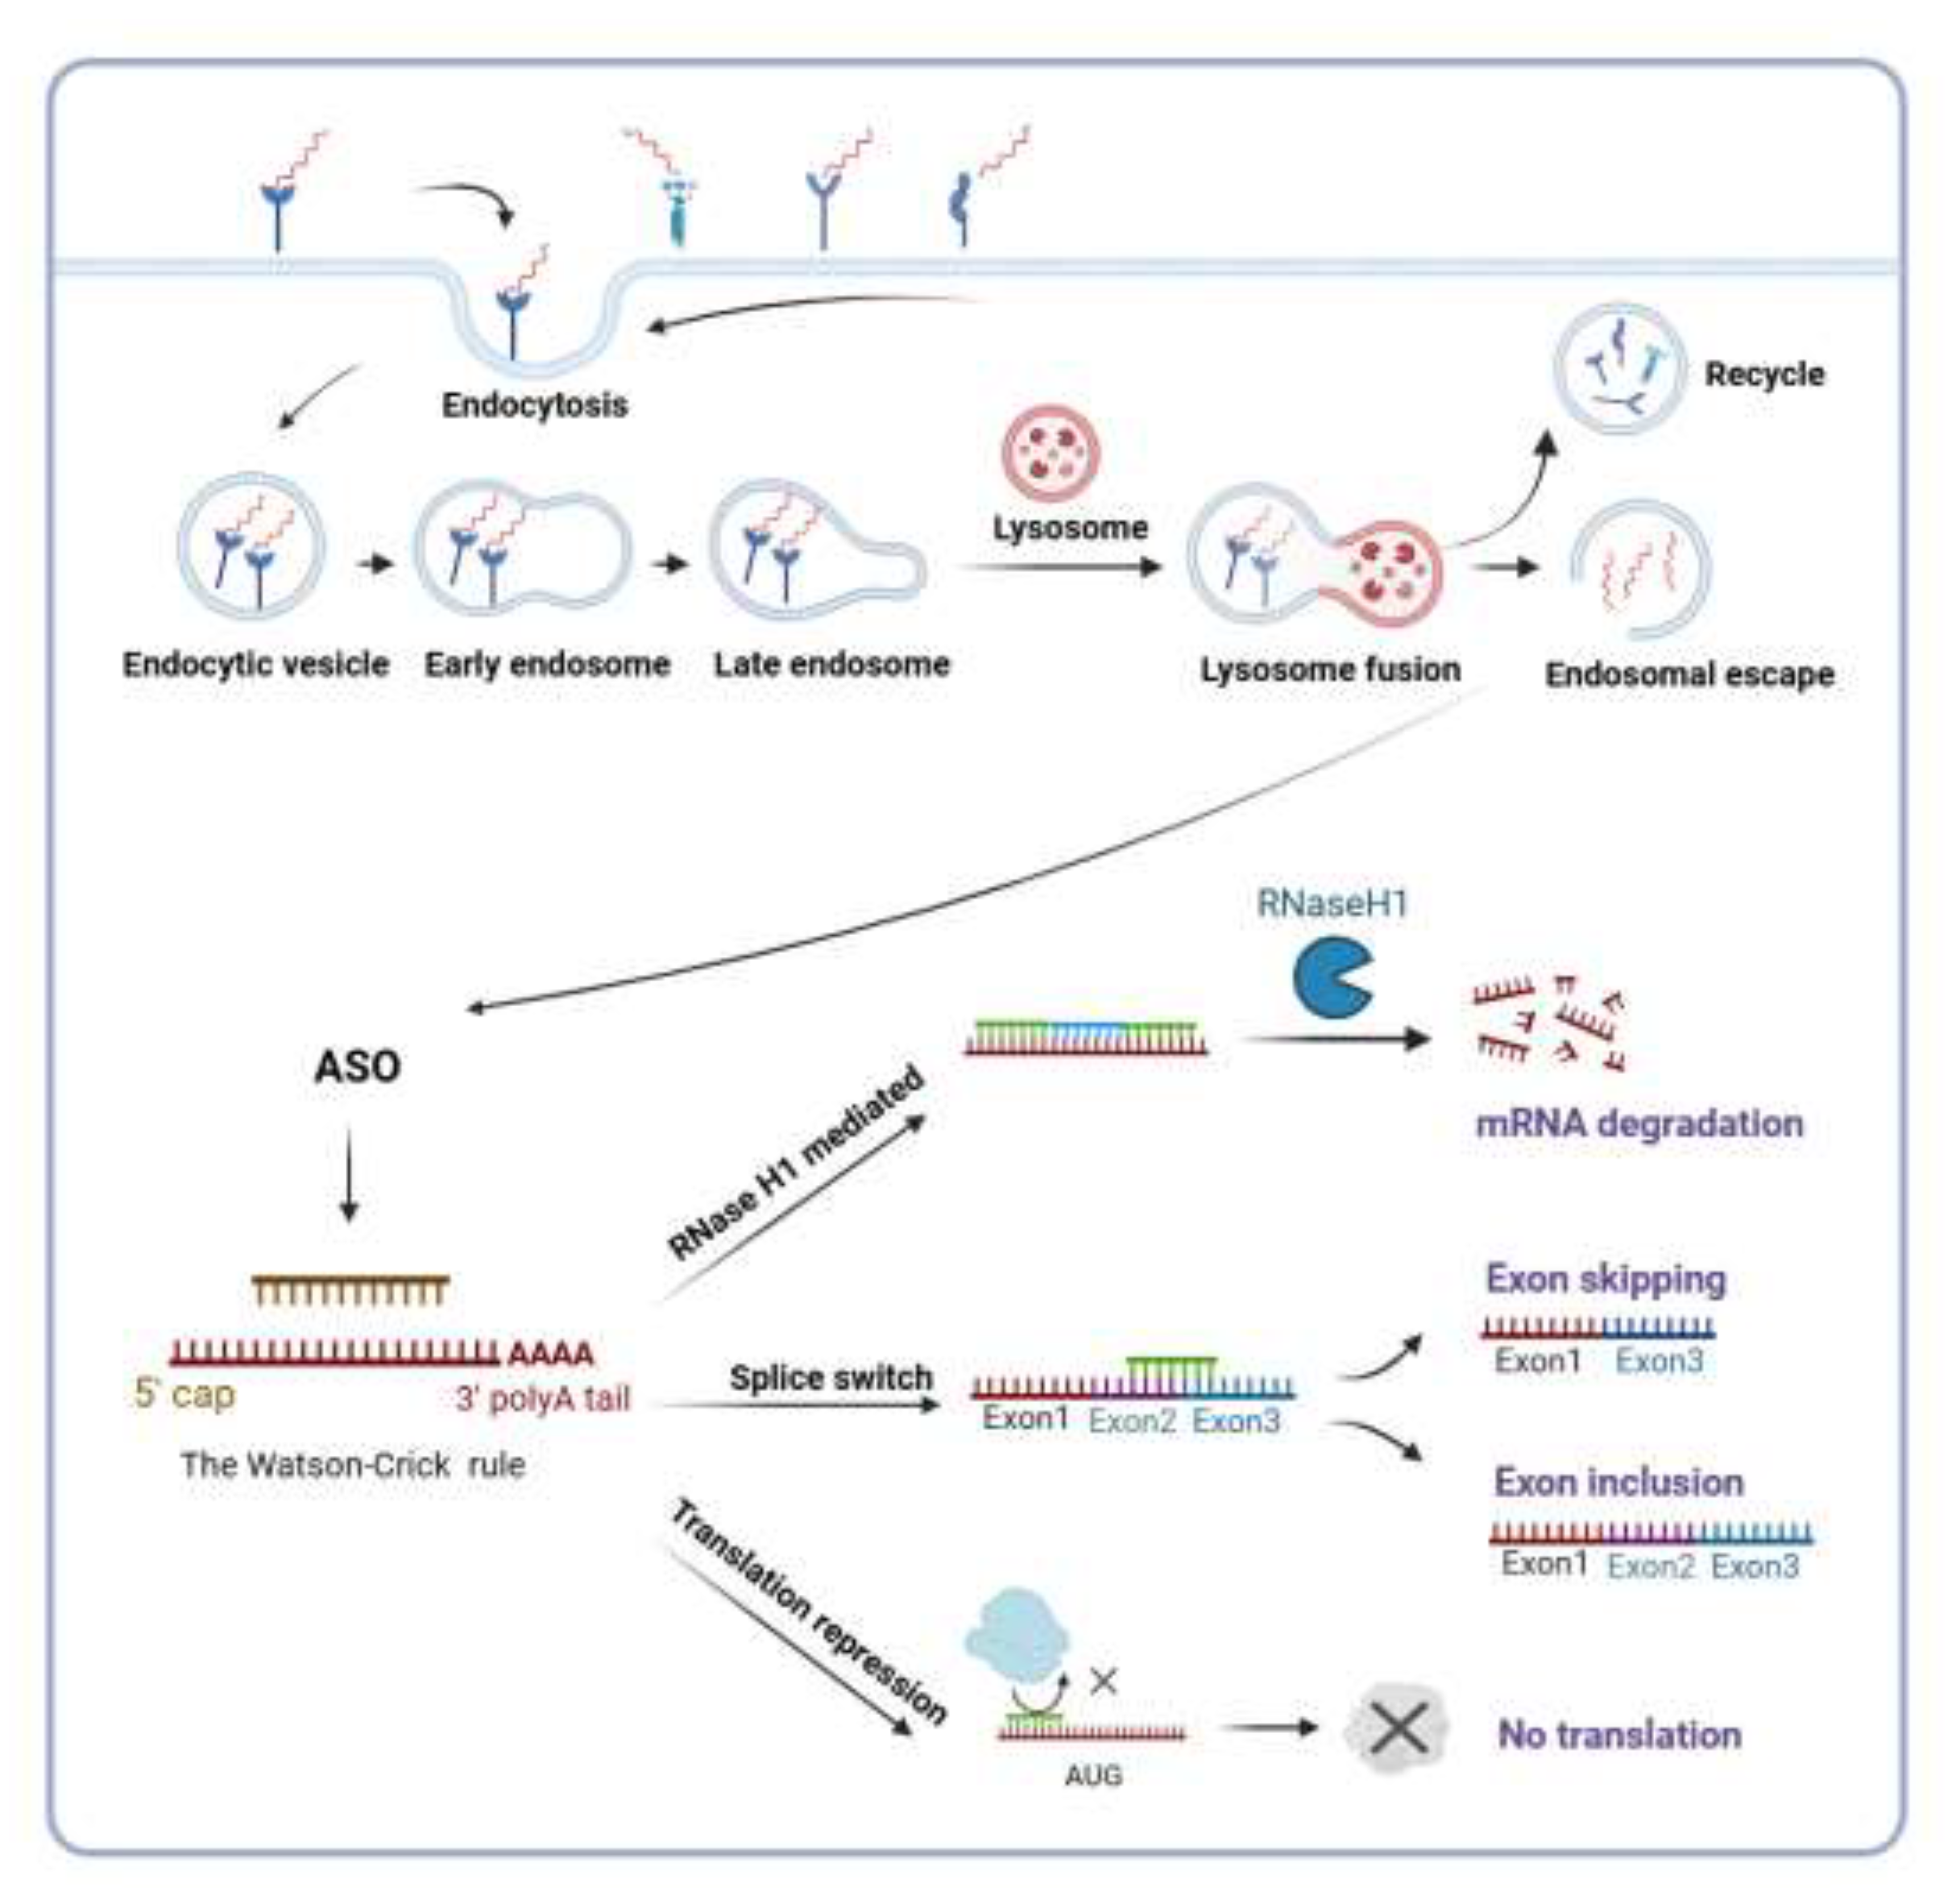
Figure 3.
Chemical modification of antisense oligonucleotides (ASOs). This figure summarizes three core modification strategies that enhance ASOs, druggability by optimizing stability, binding affinity, and safety. (a) Backbone modifications (Blue section): Target phosphodiester (PO) linkages or backbone topology (e.g., phosphorothioate [PS], phosphorodiamidate morpholino oligomers [PMOs], peptide nucleic acids [PNAs]). These modifications improve nuclease resistance, prolong in vivo half-life, and modulate protein-binding profiles while retaining or abrogating RNase H1 activity. (b) Ribose modifications (Pink section): Focus on the 2' position (e.g., 2′-O-methyl [2′-O-Me], 2′-fluoro [2′-F]) or conformational locking via bridged structures (e.g., locked nucleic acid [LNA], constrained ethyl [cEt]). These enhance hybridization stability with target mRNAs and reduce immunogenicity. (c) Base modifications (Green section): Include 5-methylcytosine (5-MeC) and C5-propynyl substitutions to mask CpG motifs (avoiding Toll-like receptor 9 activation) or strengthen base-stacking interactions, respectively, without disrupting helical geometry. The figure was created with BioRender.com. PS: Phosphorothioate; BS: boranophosphate; MP: methylphosphonate; PTE: phosphotriester; PA:phosphoramidate; PS2: phosphorodithioate; C3-amide: (3’-CH2-CO-NH-5)’; formacetal linkage: (3’-O-CH2-O-5’); Thioformacetal: replaces the 3′-sided oxygen atom with a sulfur (3’-S-CH2-O-5’); MMI: Methylene (methylimino), another nitrogen that contains an achiral four-atom linkage (3’-CH2N(CH3)-O-5’); PO: phosphodiester; PMO: phosphorodiamidate morpholino oligomer; TMO: Thiophosphoramidate morpholino oligomer; PNA: peptide nucleic acid; tcDNA: Tricyclo-DNA; SNA: serinol nucleic acid; 2ʹ-O-Me: 2ʹ-O-methyl; 2ʹ-O-MOE: 2ʹ-O-(2-methoxyethyl); 2ʹ-F: 2ʹ-fluoro; LNA: locked nucleic acid, also known as 2′,4′-bridged nucleic acids, BNA; cEt: constrained ethyl bridged nucleic acid; UNA: unlocked nucleic acid; GNA: glycol nucleic acid; ENA: ethylene-bridged nucleic acid; 5-MeC: 5-Methylcytosine; 5-MeU: 5-Methyluridine; Ψ: Pseudouridine (5-ribosyluracil); m1Ψ: N1-Methylpseudouridine.
Figure 3.
Chemical modification of antisense oligonucleotides (ASOs). This figure summarizes three core modification strategies that enhance ASOs, druggability by optimizing stability, binding affinity, and safety. (a) Backbone modifications (Blue section): Target phosphodiester (PO) linkages or backbone topology (e.g., phosphorothioate [PS], phosphorodiamidate morpholino oligomers [PMOs], peptide nucleic acids [PNAs]). These modifications improve nuclease resistance, prolong in vivo half-life, and modulate protein-binding profiles while retaining or abrogating RNase H1 activity. (b) Ribose modifications (Pink section): Focus on the 2' position (e.g., 2′-O-methyl [2′-O-Me], 2′-fluoro [2′-F]) or conformational locking via bridged structures (e.g., locked nucleic acid [LNA], constrained ethyl [cEt]). These enhance hybridization stability with target mRNAs and reduce immunogenicity. (c) Base modifications (Green section): Include 5-methylcytosine (5-MeC) and C5-propynyl substitutions to mask CpG motifs (avoiding Toll-like receptor 9 activation) or strengthen base-stacking interactions, respectively, without disrupting helical geometry. The figure was created with BioRender.com. PS: Phosphorothioate; BS: boranophosphate; MP: methylphosphonate; PTE: phosphotriester; PA:phosphoramidate; PS2: phosphorodithioate; C3-amide: (3’-CH2-CO-NH-5)’; formacetal linkage: (3’-O-CH2-O-5’); Thioformacetal: replaces the 3′-sided oxygen atom with a sulfur (3’-S-CH2-O-5’); MMI: Methylene (methylimino), another nitrogen that contains an achiral four-atom linkage (3’-CH2N(CH3)-O-5’); PO: phosphodiester; PMO: phosphorodiamidate morpholino oligomer; TMO: Thiophosphoramidate morpholino oligomer; PNA: peptide nucleic acid; tcDNA: Tricyclo-DNA; SNA: serinol nucleic acid; 2ʹ-O-Me: 2ʹ-O-methyl; 2ʹ-O-MOE: 2ʹ-O-(2-methoxyethyl); 2ʹ-F: 2ʹ-fluoro; LNA: locked nucleic acid, also known as 2′,4′-bridged nucleic acids, BNA; cEt: constrained ethyl bridged nucleic acid; UNA: unlocked nucleic acid; GNA: glycol nucleic acid; ENA: ethylene-bridged nucleic acid; 5-MeC: 5-Methylcytosine; 5-MeU: 5-Methyluridine; Ψ: Pseudouridine (5-ribosyluracil); m1Ψ: N1-Methylpseudouridine.
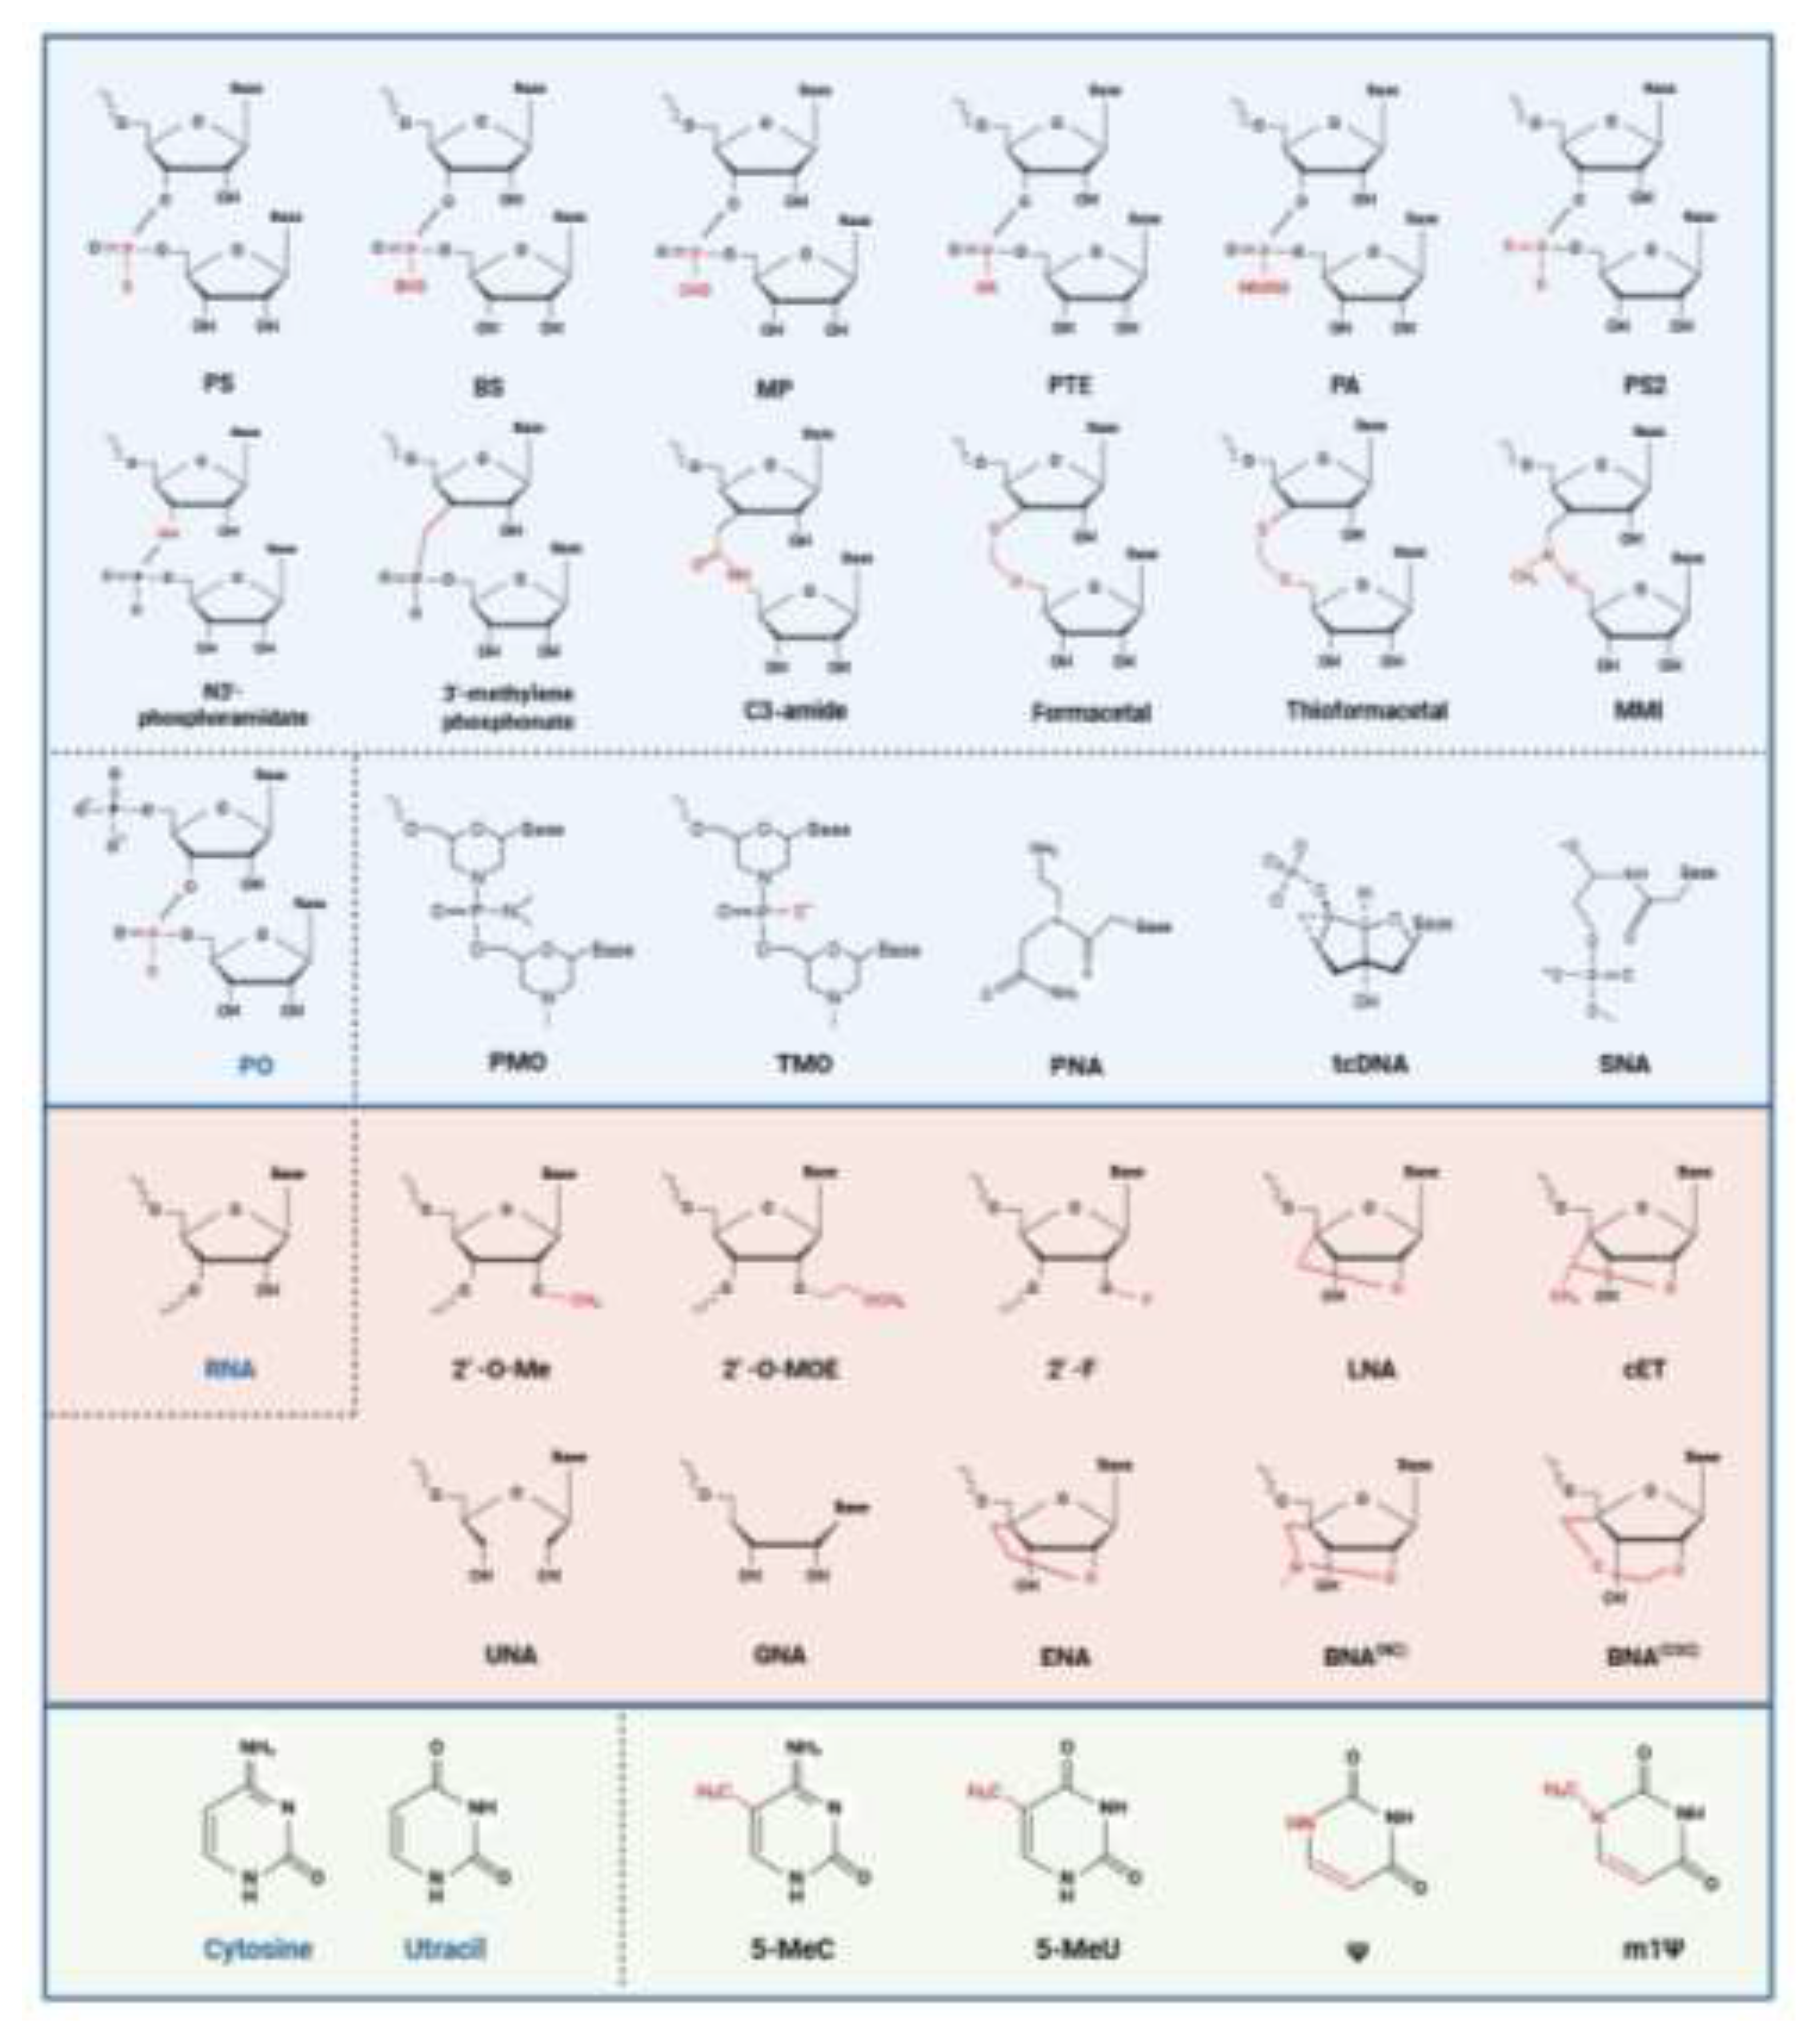
Figure 4.
Delivery strategies for antisense oligonucleotides (ASOs). This diagram outlines three key approaches to overcoming ASO transmembrane barriers and improving targeted delivery. (a) Administration routes: Clinically validated routes include intravitreal injection (for ocular diseases), intrathecal injection (for central nervous system diseases), subcutaneous injection, and intravenous injection (for systemic delivery). Route selection is guided by target tissue accessibility and the need to minimize systemic exposure. (b)Conjugate-based delivery: ASOs are covalently linked to ligands (e.g., GalNAc for hepatocyte targeting via asialoglycoprotein receptor [ASGPR]), lipophilic moieties (e.g., palmitic acid), or biomacromolecules (e.g., antibodies, cell-penetrating peptides) to enhance tissue specificity and cellular internalization (c) Non-viral carrier delivery: ASOs are encapsulated or loaded into nanocarriers such as lipid-based nanoparticles (LNPs), polymersomes, or exosomes. These carriers protect ASOs from nuclease degradation, promote endocytic uptake, and facilitate endosomal escape, thereby improving bioavailability and therapeutic efficacy. LNP: Lipid Nanoparticles; LNEs: Lipid Nanoemulsions; SLN: Solid Lipid Nanoparticles; NLC: Nanostructured Lipid Carriers; NP: Nanoparticles. The figure was created with BioRender.com.
Figure 4.
Delivery strategies for antisense oligonucleotides (ASOs). This diagram outlines three key approaches to overcoming ASO transmembrane barriers and improving targeted delivery. (a) Administration routes: Clinically validated routes include intravitreal injection (for ocular diseases), intrathecal injection (for central nervous system diseases), subcutaneous injection, and intravenous injection (for systemic delivery). Route selection is guided by target tissue accessibility and the need to minimize systemic exposure. (b)Conjugate-based delivery: ASOs are covalently linked to ligands (e.g., GalNAc for hepatocyte targeting via asialoglycoprotein receptor [ASGPR]), lipophilic moieties (e.g., palmitic acid), or biomacromolecules (e.g., antibodies, cell-penetrating peptides) to enhance tissue specificity and cellular internalization (c) Non-viral carrier delivery: ASOs are encapsulated or loaded into nanocarriers such as lipid-based nanoparticles (LNPs), polymersomes, or exosomes. These carriers protect ASOs from nuclease degradation, promote endocytic uptake, and facilitate endosomal escape, thereby improving bioavailability and therapeutic efficacy. LNP: Lipid Nanoparticles; LNEs: Lipid Nanoemulsions; SLN: Solid Lipid Nanoparticles; NLC: Nanostructured Lipid Carriers; NP: Nanoparticles. The figure was created with BioRender.com.
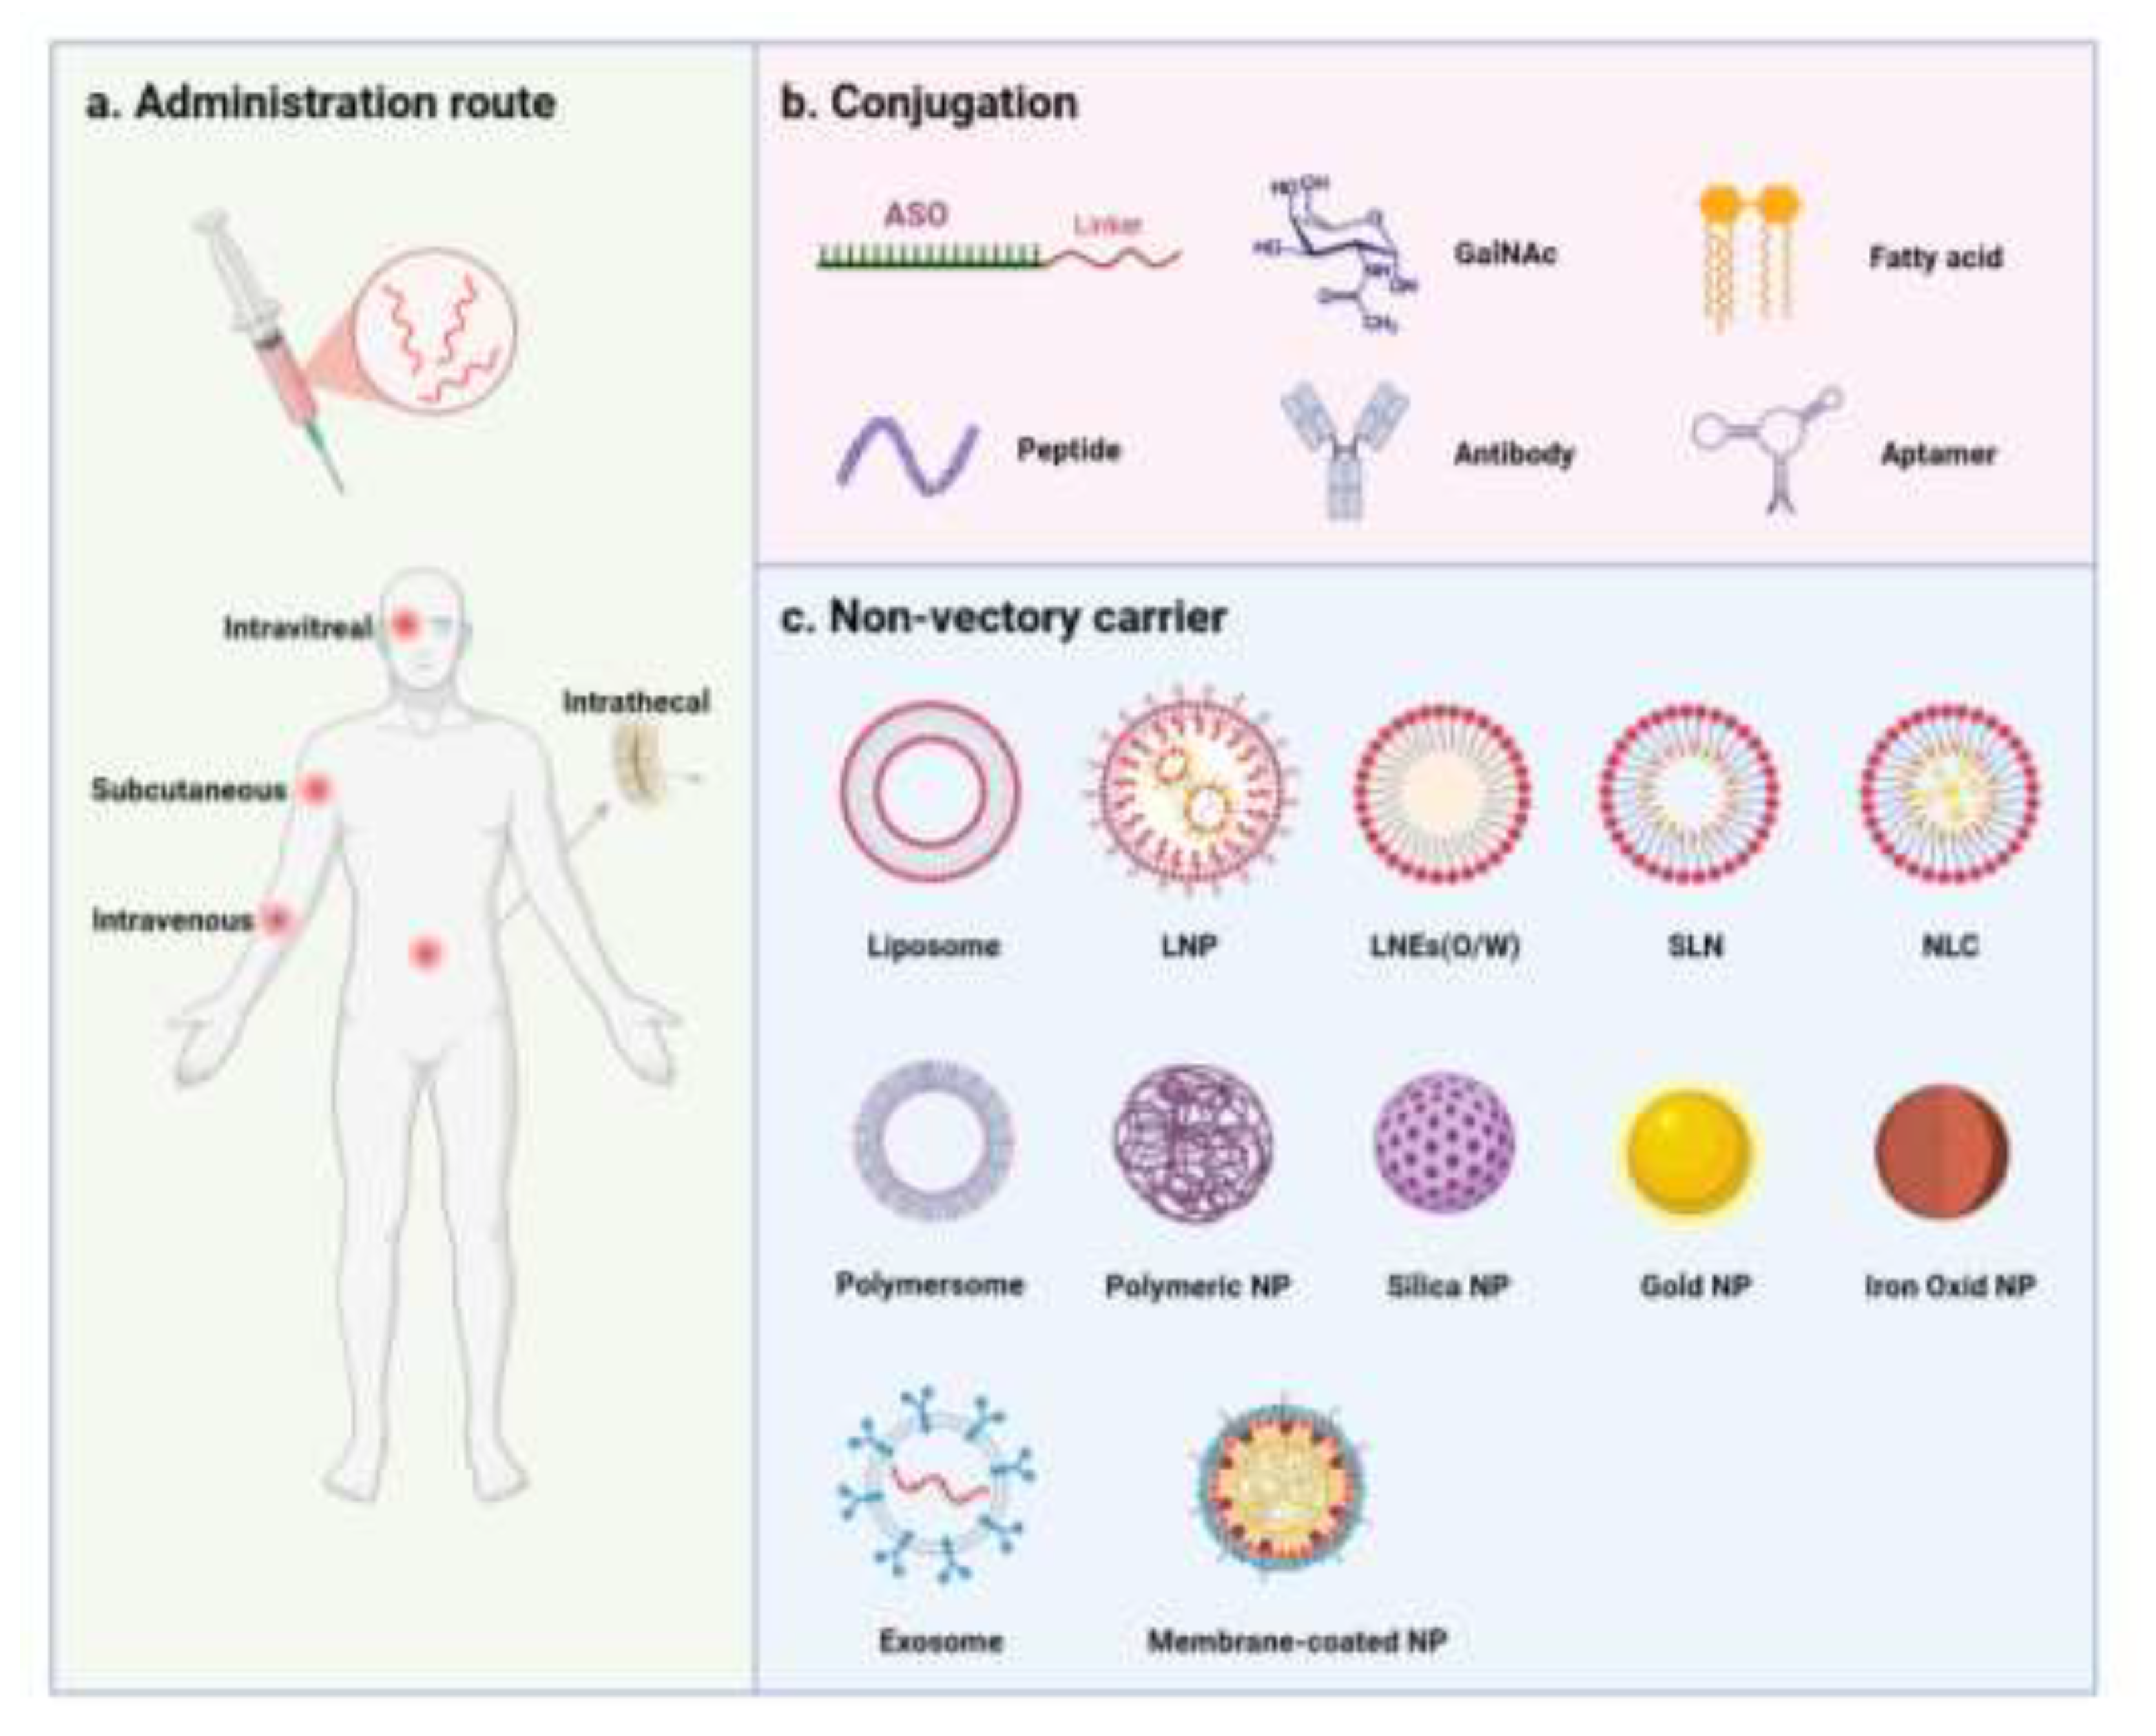

Table 1.
Overview of Approved ASOs.
| Drug Name | Trade Name | First Approval | Company | Target | Indication | Mechanism | Modification | Delivery | Delivery route | Status |
|---|---|---|---|---|---|---|---|---|---|---|
| Fomivirsen | Vitravene | 1998 | Ionis & Novartis | CMV mRNA | CMV retinitis | RNase H mediated | PS | naked | IVT | Withdrawn |
| Mipomersen | Kynamro | 2013 | Ionis & Genzyme | ApoB-100 | HoFH | RNase H mediated | 2'-MOE Gapmer | naked | SC | Withdrawn |
| Eteplirsen | Exondys 51 | 2016 | Sarepta | Dys Exon 51 | DMD | Steric blocking | PMO | naked | IV | Marketed |
| Nusinersen | Spinraza | 2016 | Ionis & Biogen | SMN2 | SMA | Steric blocking | 2'-MOE, PS | naked | IT | Marketed |
| Inotersen | Tegsedi | 2018 | Ionis & Sobi | TTR | hATTR Amyloidosis | RNase H mediated | 2'-MOE Gapmer | naked | SC | Marketed |
| Volanesorsen | Waylivra | 2019 | Ionis & Sobi | APOC3 | FCS | RNase H mediated | 2'-MOE Gapmer | naked | SC | Marketed |
| Golodirsen | Vyondys 53 | 2019 | Sarepta | Dys Exon 53 | DMD | Steric blocking | PMO | naked | IV | Marketed |
| Viltolarsen | Viltepso | 2020 | Nippon Shinyaku | Dys Exon 53 | DMD | Steric blocking | PMO | naked | IV | Marketed |
| Casimersen | Amondys 45 | 2021 | Sarepta | Dys Exon 45 | DMD | Steric blocking | PMO | naked | IV | Marketed |
| Tofersen | Qalsody | 2023 | Ionis & Biogen | SOD1 | ALS | RNase H mediated | 2'-MOE Gapmer | naked | IT | Marketed |
| Eplontersen | Wainua | 2023 | AstraZeneca & Ionis | TTR | hATTR Amyloidosis |
RNase H mediated | 2'-MOE Gapmer | GalNAc | SC | Marketed |
| Imetelstat | Rytelo | 2024 | Geron Corporation | Telomerase hTR | MDS | Telomerase inhibition | N3'-P5' Thio | Lipid | IV | Marketed |
| Olezarsen | Tryngolza | 2024 | Ionis | APOC3 | FCS | RNase H mediated | 2'-MOE Gapmer | GalNAc | SC | Marketed |
Table 2.
Discontinued Clinical-Stage ASOs.
| Phase | Drug Name / Code | Clinical Trial ID | Target | Indication | Disease Category | Mechanism | Modification | Delivery | Delivery route |
|---|---|---|---|---|---|---|---|---|---|
| III | Trabedersen (AP 12009) |
NCT00761280 NCT00431561 NCT00844064 NCT05935774 |
TGF-β2 | Glioma | Oncology & Hematology | RNase H mediated | PS | Intratumoral Perfusion | naked |
| III | Aprinocarsen (ISIS 3521/LY900003) |
NCT00017407 NCT00034268 NCT00003989 |
PKC-α | Multiple Solid Tumors | Oncology & Hematology | RNase H mediated | PS | IV | naked |
| III | Custirsen (OGX-011) |
NCT01188187 NCT01578655 |
Clusterin | CRPC | Oncology & Hematology | RNase H mediated | 2'-MOE Gapmer | IV | naked |
| III | Oblimersen (G3139/Genasense) |
NCT00024440 NCT00518895 NCT00021749 |
BCL2 | Bcl-2 Positive Malignancies | Oncology & Hematology | RNase H mediated | PS | IV | naked |
| III | Drisapersen (PRO051/GSK2402968) |
NCT01254019 NCT01153932 NCT01462292 |
DMD Exon 51 | DMD | Neuromuscular Diseases | Steric blocking | 2'-O-Me PS | SC | naked |
| III | Tominersen (RG6042/IONIS-HTTRx) |
NCT03761849 NCT03842969 NCT02519036 |
HTT | HD | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| III | Sepofarsen (QR-110) |
NCT03913143 NCT03140969 |
CEP290 | LCA10 | Ophthalmic Diseases | Steric blocking | 2'-O-Me PS | IVT | naked |
| III | Alicaforsen (ISIS 2302) |
NCT02525523 NCT00063830 NCT00048113 |
ICAM-1 | Crohn's Disease | Immunological Diseases | RNase H mediated | PS | IV/Enema | naked |
| III | Mongersen (GED-0301) |
NCT02596893 NCT02367183 |
SMAD7 | Crohn's Disease | Immunological Diseases | RNase H mediated | PS | PO | pH-dependent Coating |
| II | IONIS-DGAT2Rx | NCT03334214 | DGAT2 | Hepatic Steatosis | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | ISIS-GCGRRx | NCT02824003 NCT01885260 NCT02583919 |
GCGR | T2DM | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | ISIS-GCCRRx | NCT01968265 | GCCR | T2DM | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | ISIS-FGFR4Rx | NCT02476019 | FGFR4 | Obesity | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | CIVI-007 | NCT04164888 NCT03427710 |
PCSK9 | Hypercholesterolemia | Cardiovascular & Metabolic Diseases | RNase H mediated | LNA Gapmer | SC | GalNAc |
| II | IONIS-GHR-LRx | NCT04522180 NCT03967249 NCT03548415 |
GHR | Acromegaly | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE / cEt Gapmer | SC | GalNAc |
| II | ISIS-PTP1BRx | NCT01918865 | PTP1B | T2DM | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | IONIS-PTP1BRx (ISIS-404173) |
NCT01918865 | PTP1B | T2DM | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | Vupanorsen (ISIS 703802) |
NCT04516291 NCT03514420 NCT03360747 |
ANGPTL3 | Severe Hypertriglyceridemia / CV Risk Reduction | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| II | Atesidorsen (ATL1103) |
EUCTR2012-003147-30 ACTRN12615000289516 |
GHR | Acromegaly | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | Miravirs (SPC3649) |
NCT01200420 | miR-122 | HCV | Infectious Diseases | Anti-miR | LNA anti-miR | SC | naked |
| II | RG-101 | EudraCT:2015-001535-21 EudraCT:2015-004702-42 EudraCT:2016-002069-77 EudraCT:2013-002978-49 |
miR-122 | HCV | Infectious Diseases | Anti-miR | LNA anti-miR | SC | GalNAc |
| II | GSK3389404 (GalNAc-bepirovirsen) |
NCT03020745 | All HBV RNAs | HBV | Infectious Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| II | Donidalorsen (ISIS 721744) |
NCT04549922 | ASKCOV | COIVD-19 | Infectious Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| II | OGX-427 | NCT01829113 NCT01120470 NCT01681433 |
Hsp27 | Multiple Solid Tumors | Oncology & Hematology | RNase H mediated | 2'-MOE Gapmer | IV | naked |
| II | Danvatirsen (AZD9150) |
NCT02983578 NCT02417753 NCT03334617 NCT03794544 NCT01839604 NCT02546661 NCT02499328 NCT03527147 NCT02549651 NCT03421353 |
STAT3 | Multiple Solid Tumors | Oncology & Hematology | RNase H mediated | 2'-cEt Gapmer | IV | naked |
| II | ISIS 5132 (CGP69846A) |
NCT00002587 NCT00002588 NCT00002589 |
C-RAF-1 | Advanced Solid Tumors | Oncology & Hematology | RNase H mediated | PS | IV | naked |
| II | ISIS 2503 | NCT00004193 NCT00005594 NCT00006467 |
HRAS | Pancreatic Cancer | Oncology & Hematology | RNase H mediated | PS | IV | naked |
| II | G4460 (LR-3001) |
NCT00002592 | c-myb | CLL | Oncology & Hematology | RNase H mediated | PS | IV | naked |
| II | AEG35156 (GEM640) |
NCT00882869 | XIAP Mrna | Hepatocellular Carcinoma | Oncology & Hematology | RNase H mediated | 2'-MOE Gapmer | IV | naked |
| II | Gataparsen (LY2181308/ISIS-23722) |
NCT01107444 NCT00620321 NCT00642018 |
BIRC5 (Survivin) |
Second-line NSCLC | Oncology & Hematology | RNase H mediated | 2'-MOE Gapmer | IV | naked |
| II | Apatorsen (OGX-427) |
NCT00487786 NCT01829113 NCT02423590 NCT01454089 NCT01844817 |
HSPB1 (Hsp27) |
Multiple Solid Tumors | Oncology & Hematology | RNase H mediated | 2'-MOE Gapmer | IV | naked |
| II | QR-421a (Sepofarsen) |
NCT03780257 NCT05158296 |
USH2A exon 13 | arRP | Ophthalmic Diseases | Steric blocking | 2'-O-Me PS | IVT | naked |
| II | QR-1123 (IONIS-RHO-2.5Rx) |
NCT04123626 | RHO P23H | adRP | Ophthalmic Diseases | RNase H mediated | 2'-cEt Gapmer | IVT | naked |
| II | PGN-EDO51 | NCT06079736 | DMD Exon 51 | DMD | Neuromuscular Diseases | Steric blocking | PPMO | IV | CPP |
| II | Avicursen (ATL1102) |
ACTRN12618000936203 | CD49d | DMD | Neuromuscular Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | SRP-5051 (Vesleteplirsen) |
NCT04004065 | DMD Exon 51 | DMD | Neuromuscular Diseases | Steric blocking | PPMO | IV | CPP |
| II | IONIS-PKKRx | NCT03254362 | PKK | Chronic Migraine | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | WVE-120101 | NCT03225833 NCT04617847 |
mHTT SNP1 | HD | Neurological Diseases | RNase H mediated | PN Chemistry | IT | naked |
| II | WVE-120102 | NCT03225846 NCT04617860 |
mHTT SNP1 | HD | Neurological Diseases | RNase H mediated | PN Chemistry | IT | naked |
| II | ION-827359 (IONIS-ENaC-2.5Rx) |
NCT03647228 | SCNN1A/B/G | Cystic Fibrosis | Respiratory Diseases | RNase H mediated | 2'-cEt Gapmer | INH | naked |
| II | Fesomersen (ISIS 416858) |
NCT03358030 NCT02553889 |
Factor XI | Thromboprophylaxis / Anticoagulation | Hematological Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
| II | QR-313 (WNG-313) |
NCT03605069 | COL7A1 Exon73 | RDEB | Genodermatoses | Steric blocking | 2'-O-Me PS | TOP | naked |
| I/II | RG125 (AZD4076) |
NCT02826525 NCT02612662 |
miR-103/107 | T2DM with NAFLD / NASH | Cardiovascular & Metabolic Diseases | Anti-miR | LNA anti-miR | SC | GalNAc |
| I/II | Cavrotolimod (AST-008) |
NCT03684785 NCT03086278 |
TLR9 | PD-1 Resistant Tumors | Oncology & Hematology | Immune Activation | SNA | SC | naked |
| I/II | AZD5312 | NCT02144051 NCT03300505 |
AR | CRPC | Oncology & Hematology | RNase H mediated | 2'-cEt Gapmer | IV | naked |
| I/II | BIIB105 (ION541) |
NCT04494256 | ATXN2 | ALS(ATXN2) | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| I | EZN-2968 | NCT00466583 NCT01120288 |
HIF-1α | Solid Tumors or Lymphoma | Oncology & Hematology | RNase H mediated | LNA Gapmer | IV | naked |
| I | RO7070179 | NCT02564614 | HIF1A | HCC | Oncology & Hematology | RNase H mediated | Unknown | IV | naked |
| I | CDK-004 | NCT05375604 | STAT6 | HCC | Oncology & Hematology | RNase H mediated | Unknown | IV | exosome |
| I | Radavirsen (AVI-7100) |
NCT01747148 | M1/M2 | Influenza A Virus | Infectious Diseases | Steric blocking | PMO | IV | PMOplus |
| I | RO7062931 | NCT03038113 NCT03505190 |
All HBV RNAs | HBV | Infectious Diseases | RNase H mediated | LNA Gapmer | SC | GalNAc |
| I | ALG-020572 | NCT05001022 | All HBV RNAs | HBV | Infectious Diseases | RNase H mediated | BNA Gapmer | SC | GalNAc |
| I | BIIB078 (IONIS-C9Rx) |
NCT03626012 NCT04288856 |
C9orf72 | ALS/FTD | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| I | WVE-004 | NCT04931862 NCT05683860 |
C9orf72 | ALS/FTD | Neurological Diseases | RNase H mediated | PN Chemistry | IT | naked |
| I | NIO752 | NCT04539041 | TAU | PSP | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| I | ISIS 388626 | NCT00836225 | SGLT2 | T2DM & Obesity | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | naked |
Table 3.
Potential ASOs in Ongoing Clinical Trials.
| Phase | Drug Name / Code | Clinical Trial ID | Target | Indication | Disease Category | Mechanism | Modification | Delivery | Delivery route |
|---|---|---|---|---|---|---|---|---|---|
| III | Zilganersen (ION373) |
NCT04849741 | GFAP | Alexander Syndrome | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| III | ION582 (BIIB121) |
NCT06914609 NCT05127226 |
UBE3A-ATS | Angelman Syndrome | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| III | GTX-102 (Apazunersen) |
NCT06617429 NCT07157254 NCT04259281 |
UBE3A-ATS | Angelman Syndrome | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| III | ION363 (Jacifusen,Ulefnersen) |
NCT04768972 | FUS | ALS (FUS) | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| III | Zorevunersen (STK-001) |
NCT06872125 NCT04740476 NCT04442295 |
SCN1A | Dravet Syndrome | Neurological Diseases | TANGO | 2'-MOE ODN | IT | naked |
| III | Eteplirsen (approved LTE) |
NCT02420379 NCT02286947 |
DMD Exon 51 | DMD | Neuromuscular Diseases | Steric blocking | PMO | IV | naked |
| III | Bepirovirsen (GSK3228836) |
NCT05630820 NCT05630807 NCT04449029 NCT04954859 NCT04676724 NCT04544956 NCT02981602 |
All HBV RNAs | HBV;CHB | Infectious Diseases | RNase H mediated Immune Activation |
2'-MOE Gapmer | SC | naked |
| III | AHB-137 | NCT07246889 NCT07146100 NCT05717686 NCT06550128 NCT07069569 NCT06115993 |
All HBV RNAs | HBV | Infectious Diseases | RNase H mediated Immune Activation |
Med-Oligo™ | SC | naked |
| III | NEXAGON (Lufepirsen) |
NCT05966493 NCT04081103 NCT01165450 |
Connexin 43 | PCED | Ophthalmic Diseases | Steric blocking | ODN | Eye Gel | naked |
| III | Sefaxersen (IONIS-FB-LRx, RO7434656) |
NCT05797610 NCT03815825 NCT04014335 |
Complement Factor B | IgA Nephropathy (IgAN) | Immunological Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| III | Pelacarsen (TQJ230) |
NCT04023552 NCT06875973 NCT05305664 NCT05900141 NCT06267560 NCT06813911 NCT05646381 NCT03070782 |
LPA | Lp(a), CVD | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| III | Olezarsen | NCT05079919 NCT05552326 NCT05681351 |
APOC3 | sHTG– CORE | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| III | Olezarsen | NCT05355402 NCT05610280 NCT03385239 NCT02900027 |
APOC3 | Hypertriglyceridemia w/ ASCVD or High CV Risk | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| III | Eplontersen | NCT04136171 | TTR | ATTR-CM | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| III | Olezarsen (approved LTE) |
NCT05185843 | APOC3 | FCS | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| III | Donidalorsen (approved LTE) |
NCT05139810 | PKK | HAE | Immunological Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| II | AZD2693 (ION839) |
NCT05809934 (CTR20232127) |
PNPLA3 | MASH | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| II | IONIS-AGT-LRx | NCT03714776 NCT04083222 |
AGT | Resistant Hypertension | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| II | ION224 (IONIS-DGAT2Rx) |
NCT03334214 NCT04932512 |
DGAT2 | MASH with Fibrosis | Cardiovascular & Metabolic Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| II | QR-421a (Ultevursen) |
NCT06627179 | USH2A exon 13 | arRP | Ophthalmic Diseases | Steric blocking | 2'-O-Me PS | IVT | naked |
| II | Fesomersen (BAY2976217) |
NCT04534114 | Factor XI | Thromboprophylaxis / Anticoagulation | Hematological Diseases | RNase H mediated | 2'-MOE Gapmer | SC | GalNAc |
| II | AZD2373 (Opemalirsen) |
NCT06824987 | APOL1 | AMKD | Kidney Disease | RNase H mediated | 2'-cEt Gapmer | SC | naked |
| II | OT-101 | NCT06079346 NCT05425576 |
TGF-β2 | PDAC; MPM | Oncology & Hematology | RNase H mediated | PS | Intratumoral Perfusion | naked |
| II | BP1001 (Prexigebersen) |
NCT02781883 | Grb-2 | AML、ALL、CML-BP、MDS | Oncology & Hematology | RNase H mediated | P-ethoxy-DNA | IV | Liposome |
| II | Danvatirsen (AZD9150) |
NCT05814666 | STAT3 | HNSCC | Oncology & Hematology | RNase H mediated | 2'-cEt Gapmer | IV | naked |
| II | BIIB080 (IONIS-MAPT Rx) |
NCT05399888 NCT03186989 |
MAPT | AD | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| II | WVE-003 | NCT05032196 | mHTT SNP3 | HD | Neurological Diseases | RNase H mediated | PN Chemistry (Stereopure) | IT | naked |
| II | WVE-N531 | NCT04906460 | Dystrophin Exon 53 | DMD | Neuromuscular Diseases | Steric blocking | PN Chemistry (Stereopure) | IV | naked |
| I/II | Elsunersen (PRAX-222) |
NCT05737784 | SCN2A | SCN1A-Associated DEE | Neuromuscular Diseases | RNase H mediated | 2'-MOE gapmer | IT | naked |
| I/II | DYNE-251 | NCT05524883 | Dys Exon 51 | DMD | Neuromuscular Diseases | Steric blocking | PMO | IV | Fab-PMO(AOC) |
| I/II | AOC-1044 (del-zota) |
NCT05670730 | Dys Exon 44 | DMD | Neuromuscular Diseases | Steric blocking | PMO | IV | Fab-PMO(AOC) |
| I/II | ISTH0036 | NCT02406833 | TGF-β2 | POAG | Ophthalmic Diseases | RNase H mediated | LNA Gapmer | IVT | naked |
| I | ASOTARI | NCT06451172 | Essential genes for bacterial | Antibiotic-resistant bacterial keratitis | Ophthalmic & Infectious Diseases | Trojan Horse Strategy | PNA | Eye Drops | GP-SiNPs-asPNA |
| I | STK-002 | ISRCTN41725621 | OPA1 | ADOA | Ophthalmic Diseases | TANGO | 2'-MOE Gapmer | IVT | naked |
| I | NIO752 | NCT05469360 NCT06372821 |
TAU | AD | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| I | ION356 | NCT05786433 | PLP1 | PMD | Neurological Diseases | RNase H mediated | 2'-MOE / cEt Gapmer | IT | naked |
| I | ION716 | NCT06249918 | Prion Protein | CJD | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| I | AMX0114 | NCT06665165 | CAPN2 | ALS (CAPN2) | Neurological Diseases | RNase H mediated | 2'-MOE Gapmer | IT | naked |
| I | Atipeksen | NCT07215416 | ATM Exon 53 | A-T | Neurological Diseases | Steric blocking | 2'-MOE PS | IT | naked |
| I | BP1002(Liposome) | NCT04072458 NCT05190471 |
Bcl-2 | Bcl-2 Positive Malignancies | Oncology & Hematology | RNase H mediated | P-ethoxy-DNA | IV | Liposome |
| I | Danvatirsen (AZD9150) |
NCT03819465 | STAT3 | NSCLC | Oncology & Hematology | RNase H mediated | 2'-cEt Gapmer | IV | naked |
| I | Danvatirsen (AZD9150) |
NCT05986240 | STAT3 | AML / MDS | Oncology & Hematology | RNase H mediated | 2'-cEt Gapmer | IV | naked |
| I | OT-101 | NCT06579196 | TGF-β2 | NSCLC | Oncology & Hematology | RNase H mediated | PS | Intratumoral Perfusion | naked |
Table 4.
ASOs for Individualized Therapy.
| NCT Number | Target | Drug Name / Code | Indication | Sponsor | status |
|---|---|---|---|---|---|
| NCT07197268 | ASXL3 | nL-ASXL3-001 | BRS | n-Lorem Foundation | Active |
| NCT07215416 | ATM | ASO targeting ATM | A-T | academic institution | Active |
| NCT06706388 | ATN1 | nL-ATN1-002 | DRPLA | n-Lorem Foundation | Active |
| NCT07084311 | ATN1 | nL-ATN1-002 | DRPLA | n-Lorem Foundation | Active |
| NCT07221760 | ATN1 | nL-ATN1-001 | DRPLA | n-Lorem Foundation | Not yet recruiting |
| NCT06392126 | CHCHD10 | nL-CHCHD-001 | ALS (CHCHD10 related) | n-Lorem Foundation | Active |
| NCT06977451 | CHCHD10 | nL-CHCHD-001 | ALS (CHCHD10 related) | n-Lorem Foundation | Active |
| NCT07095686 | CHCHD10 | nL-CHCHD-001 | ALS (CHCHD10 related) | n-Lorem Foundation | Enrolling |
| NCT06565572 | FLVCR1 | nL-FLVC-001 | PCARP | academic institution | Enrolling |
| NCT06816498 | LMNB1 | nL-LMNB1-001 | ADLD | n-Lorem Foundation | Active |
| NCT07197294 | MAPK8IP3 | nL-MAPK8-001 | NEDBA | n-Lorem Foundation | Active |
| NCT07177196 | PRPH2 | nL-PRPH2-001 | Retinal Dystrophy | n-Lorem Foundation | Active |
| NCT06314490 | SCN2A | nL-SCN2A-002 | SCN2A-Related Disorders | academic institution | Active |
| NCT07095712 | TARDBP | nL-TARD-001 | ALS (TDP-43 related) | n-Lorem Foundation | Active |
| NCT07222371 | TUBB4A | nL-TUBB4-001 | Leukodystrophy | academic institution | Active |
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (http://creativecommons.org/licenses/by/4.0/).
Copyright: This open access article is published under a Creative Commons CC BY 4.0 license, which permit the free download, distribution, and reuse, provided that the author and preprint are cited in any reuse.