
Submitted:
19 September 2026
Posted:
20 September 2026
You are already at the latest version
Abstract
The Pyraloidea are among the largest superfamilies of Lepidoptera, yet their distribution in the eastern Mediterranean is documented unevenly. Light-trapping was carried out on 54 nights between 2008 and 2024 at 45 localities in the districts of Erdemli and Mezitli, Mersin Province, southern Türkiye, along an elevational gradient from 150 to 1800 m a.s.l. The survey yielded 492 occurrence records of 1330 specimens belonging to 161 species in 91 genera; the Pyralidae are represented by 78 species and the Crambidae by 83, and the largest subfamilies are the Phycitinae (61 species), the Crambinae (23) and the Spilomelinae (22). Eighty species are reported for the first time from Mersin Province, the assessment being made against the national catalogue, two annotated lists for the district of Anamur, an unpublished doctoral thesis on the region and the applied entomological literature. Nomenclature was checked species by species against the Global Information System on Pyraloidea, which altered 28 entries relative to the source material and included five changes of generic placement and one synonymy. Ten of the species were described from Anatolian type localities. Species composition became increasingly dissimilar with increasing elevational distance between sampling events (Spearman ρ = 0.187, p < 0.001), an effect independent of season, and 94% of the dissimilarity between assemblages was attributable to species replacement rather than to nestedness; no significant relationship between elevation and species richness per night was found once overdispersion was accounted for. Sample-based rarefaction and the Chao2 estimator indicate that about three-quarters of the pyraloid fauna likely to be present has been recorded. Neither district contains a protected area. The occurrence data are published in Darwin Core format.
Keywords:
Pyralidae
; Crambidae
; faunistics
; new provincial records
; light trap
; Taurus Mountains
; elevational gradient
; species turnover
; Darwin Core
1. Introduction
The Pyraloidea are among the largest superfamilies of Lepidoptera and one of the most consequential for human affairs. The group includes stored-product pests, defoliators of forest and orchard trees, borers of cereals and reeds, and a considerable number of species whose larvae are restricted to single host genera; it also includes the only lepidopteran lineage with truly aquatic larvae. Adults come readily to light, so that the superfamily is well represented in trap catches, yet in much of the eastern Mediterranean the group remains far less thoroughly surveyed than the butterflies or the larger moths.
Türkiye occupies a position of unusual interest for the group. The country lies at the meeting point of the Euro-Siberian, Mediterranean and Irano-Turanian regions, and its Pyraloidea fauna is correspondingly rich: 672 species were listed in the most recent national catalogue [1], and both new species and new provincial records continue to be described: Elegia feminina was described from Anamur, in the province treated here, as recently as 2020 [12], and a single season of light-trapping in Köprülü Canyon added 72 species to the list for Antalya Province [35]. Much of the older material was collected in the nineteenth century by travelling naturalists, and a substantial number of pyraloid species were described from Anatolian type localities; ten of the species reported below fall into this category.
Research on the Turkish Pyraloidea has followed two rather separate paths, and neither has produced much in the way of regional inventory. The larger body of work is applied, and concerns single species of economic importance: Ectomyelois ceratoniae on figs, pomegranates and citrus, Cryptoblabes gnidiella on pomegranate and persimmon, Hellula undalis on brassicas, Ostrinia nubilalis and the introduced Chilo partellus on maize, Cydalima perspectalis on box, Loxostege sticticalis on forage crops [2,3,4,5,6]. These papers record biology, damage and control, and the localities they give are those of the crop rather than of the fauna. The faunistic literature is smaller and its coverage patchy: 22 species from Hatay [7], 15 Crambidae from Gaziantep [8], 193 taxa from a single district of Bitlis [9], 92 species from Adana, Mersin and Osmaniye in an unpublished thesis [10]. Set against the 672 species listed for the country as a whole [1], these figures show how little of Türkiye has been surveyed with a light trap for this superfamily.
Mersin Province, on the Mediterranean coast of southern Türkiye, is a favourable area for such a fauna. Within a short horizontal distance the land rises from the Çukurova plain to the southern slopes of the central Taurus range, so that Mediterranean lowland, maquis, coniferous forest and karstic upland grassland occur in close proximity. Despite this, the pyraloid fauna of the province has been documented unevenly. The most substantial recent work concerns the district of Anamur, at the western end of the province, where two annotated lists have appeared [11,12]; the districts of the central and eastern parts of the province have received far less attention, and no faunistic work devoted to Erdemli or Mezitli appears to have been published before the theses on which the present paper is based.
The present paper reports the results of light-trapping carried out in the districts of Erdemli and Mezitli between 2008 and 2024. The material derives in part from four Master’s theses carried out at Mersin University, two on the Pyralidae and two on the Crambidae of the districts of Erdemli and Mezitli [13,14,15,16], and in part from additional collections held in the Entomological Research Laboratory (ENTOLAB) of Mersin University. Together these yield 492 occurrence records of 1,330 specimens, representing 161 species in 91 genera, collected on 54 nights at 45 localities between 150 and 1,800 m a.s.l. The Pyralidae are represented by 78 species and the Crambidae by 83; the largest subfamilies are the Phycitinae (61 species), the Crambinae (23) and the Spilomelinae (22).
Three aims are pursued here. The first is to provide an annotated checklist of the Pyraloidea of two districts that span the whole elevational range from the Mediterranean plain to the subalpine belt of the central Taurus. The second is to establish, against the several sources now available, which of the species are new to the province. The third is to describe how the fauna is distributed along the gradient, and to assess how completely it has been sampled.
2. Materials and Methods
The study was carried out in the districts of Erdemli and Mezitli, Mersin Province, on the Mediterranean coast of southern Türkiye. Both districts extend from the coastal plain northwards into the southern slopes of the central Taurus range, so that a short horizontal distance spans a wide altitudinal range. Sampling localities lie between 150 and 1,800 m a.s.l. and between 36°31′21″ and 36°58′31″ N and between 34°04′06″ and 34°29′15″ E.
The region falls within the Mediterranean bioclimatic zone, with mild wet winters and hot dry summers. The vegetation changes with elevation from irrigated cultivation and coastal scrub on the plain, through Mediterranean maquis and Pinus brutia woodland at intermediate elevations, to an oro-Mediterranean belt of Pinus nigra, Cedrus libani and Abies cilicica with open karstic grassland above. This follows the two-formation scheme of Atalay [17] for the vegetation of the region.
2.2. Sampling
Adult moths were collected at light on 54 nights between 2008 and 2024 (3 nights in 2008, 4 in 2009, 7 in 2012, 6 in 2013, 4 in 2014, 8 in 2021, 9 in 2022, 10 in 2023 and 3 in 2024). Sampling was concentrated in the warm season: 224 records derive from July, 122 from August, 56 from September, 36 from June and 30 from May, with smaller numbers from April, October and November.
At each locality the equipment was set up before dusk; collecting began at nightfall and continued until approximately 02:00, giving five to six hours per night. A 160 W mercury-vapour lamp (Philips ML, E27; Koninklijke Philips N.V., Amsterdam, The Netherlands) was operated against a white screen measuring 2 × 3 m. A second, ultraviolet source was run simultaneously a short distance away, so that the two lights did not overlap: a fluorescent floodlight in which the standard tube had been replaced with an 18 W blacklight-blue tube (BLB T8, JB-Light). Power for both was supplied by a portable petrol generator of 1000 W. One locality was worked per night. Specimens were killed in ethyl acetate vapour and transported in paper envelopes. In the laboratory they were held at −45 °C in a deep freezer (Uğur) to eliminate parasites, then pinned with entomological pins, set with the wings spread on setting boards using tracing paper, and dried in a drying oven (Nüve EN 500) at 65 °C for 24 h. Dried specimens were provided with printed labels and are deposited in the Entomological Research Laboratory (ENTOLAB), Mersin University.
Coordinates were obtained in the field with a Garmin GPSMAP 64sx receiver (nominal accuracy ±5 m) and are reported in decimal degrees on the WGS84 datum. Sampling points lying within 500 m of one another were treated as a single locality, and their coordinates averaged; the coordinate uncertainty given for each locality is derived from the spread of its constituent points and is 250 m for single-point localities and up to 850 m for the two clustered ones. This yielded 45 localities, 27 in Erdemli and 18 in Mezitli, distributed among elevational belts as follows: 8 below 400 m, 14 between 401 and 800 m, 8 between 801 and 1,200 m and 15 above 1,200 m.
2.3. Identification and Nomenclature
Specimens were identified from external characters, principally wing pattern, wing shape and labial palp structure, and by comparison with named material in ENTOLAB. Two works served as the principal identification sources, between them covering 159 of the 161 species reported here. Slamka’s Pyraloidea of Europe was used for the Pyralinae, Galleriinae and Odontiinae [18], the Crambinae and Schoenobiinae [19], the Pyraustinae and Spilomelinae [20] and the Phycitinae [21]; the last of these covers the Cryptoblabini and part of the Phycitini, and a small number of phycitine species in the present list fall outside its scope. Goater, Nuss and Speidel [22] was used for the Scopariinae, Evergestinae and Schoenobiinae, which are not treated in the Slamka series. The two Glaphyriinae recorded here, Hyperlais dulcinalis and Prochoristis crudalis, are covered by neither work; they were determined by comparison with identified material figured on Lepiforum, Lepidoptera.eu and UKMoths, and both should be regarded as requiring confirmation. Genitalic dissection was not undertaken and no molecular work was carried out.
Nomenclature and generic placement follow the Global Information System on Pyraloidea (GlobIZ) [23], consulted for every species in the list. Two conventions are applied. First, GlobIZ retains the original spelling of species-group names without applying gender agreement with the generic name, and this usage is followed here, so that combinations such as Catoptria acutangulellus, Euchromius bella, Donacaula niloticus and Pseudobissetia terrestrellus depart from the spellings used in some regional literature. Second, the conventional square brackets are retained for the anonymous 1775 work of [Denis & Schiffermüller] and for dates inferred from works published in parts, where GlobIZ gives a range rather than a single year (Catoptria mytilella (Hübner, [1805]), Anania perlucidalis (Hübner, [1809]), Thopeutis cicatricella (Hübner, [1824])).
Checking every name against GlobIZ altered 28 entries relative to the original theses. Five species proved to belong to genera other than those under which they had been listed: Laodamia combustella (as Alophia), Chrysocramboides craterella (as Chrysocrambus), Ectomyelois ceratoniae (as Apomyelois), Myelopsis tetricella (as Episcythrastis) and Thopeutis cicatricella (as Friedlanderia). One name, Pyrausta neglectalis Caradja, 1916, is treated in GlobIZ as a synonym of P. virginalis Duponchel, 1832 [24], and the two entries were accordingly merged. The remaining changes concern misspellings, authorship, date and the use of parentheses. Because much of the regional literature uses the earlier combinations, both are given in the checklist.
2.4. Provisional Identifications
Records of taxa that cannot be separated with confidence on external characters alone are treated as provisional. This applies to the genera Cadra, Delplanqueia, Ephestia, Epischnia, Homoeosoma, Pempelia, Pempeliella and Phycitodes (Pyralidae: Phycitinae) and to Eudonia and Scoparia (Crambidae: Scopariinae). In these groups wing-pattern variation within a species commonly exceeds the differences between species and reliable determination requires examination of the genitalia. Thirty of the 161 species (18.6%) fall into this category, accounting for 84 records (17.1%) and 218 specimens (16.4%). They are flagged in the checklist and are excluded from any statement of first provincial record. The effect is uneven: it is most consequential in Phycitodes (five species, 71 specimens) and Eudonia (five species, 77 specimens), where long series were assigned to single species on external appearance alone; it is least consequential in Cadra, Ephestia, Homoeosoma, Delplanqueia and Pempeliella, where the material amounts to one or two specimens per species. Because all material is preserved as vouchers in ENTOLAB, these identifications remain open to verification.
2.5. Locality Data and Cartography
Sampling localities are listed in Table 1 and mapped in Figure 1. Coordinates were recorded in decimal degrees on the WGS84 datum (EPSG:4326) with a Garmin GPSMAP 64sx receiver (Garmin Ltd., Olathe, KS, USA; nominal accuracy ±5 m). Localities are numbered 01–45 in Table 1 and in Figure 1; in the occurrence dataset the same localities carry the identifiers L01–L45, the prefix being retained so that the locationID field remains alphanumeric and cannot be read as a number.
Figure 1 was produced with a Python script. Python 3.12.3 was used with GeoPandas 1.1.4 [25] for vector data handling, Shapely 2.1.2 (GEOS 3.13.1) for geometric operations, pyproj 3.7.2 (PROJ 9.5.1) for coordinate transformation and Matplotlib 3.10.8 [26] for rendering; NumPy 2.4.4 [27] and pandas 3.0.2 [28] were used for tabular processing.
All layers were transformed from EPSG:4326 to the projected coordinate reference system UTM zone 36N (EPSG:32636, WGS84) before drawing, so that the scale bar and all distances on the map are metric and undistorted at this extent. The north arrow indicates true (geographic) north. The ten localities of the eastern Mezitli cluster remain too close to separate at the scale of the main panel and are shown enlarged in Figure 1c.
Symbol colour denotes the elevational belt, following the four-class sequential ColorBrewer scheme YlGnBu [29,30]. Provincial and district boundaries and the coastline were taken from the openly licensed administrative boundary dataset for Türkiye distributed by ttezer [31]. Panel (a) uses the same dataset dissolved to the national outline; the axis of the Taurus range drawn in that panel is schematic and is shown only to locate the three conventional subdivisions of the range relative to the study area.
2.6. Data Analysis
A night at one locality is treated as one sampling unit, giving 54 units. Sample-based rarefaction curves were computed by randomising the order of the units 1000 times and averaging the accumulated number of species at each step, with a 95% band taken as ±1.96 standard deviations. Total richness was estimated with the incidence-based Chao2 estimator [32] and, for comparison, with the abundance-based Chao1.
The relationship between elevation and the number of species recorded per night was examined with generalised linear models. Because the counts were strongly overdispersed (Pearson dispersion 3.2 for the analysed subset and 4.6 for the whole dataset), a negative binomial model was fitted rather than a Poisson one, with elevation and sampling month as covariates and, in a second model, the district as a further term.
Compositional turnover was measured as the Sørensen dissimilarity between all pairs of sampling events, and related to the elevational distance and to the difference in sampling month between them by Spearman rank correlation. Turnover was also compared within and between elevational belts with a Mann–Whitney test. Total dissimilarity was partitioned into its turnover and nestedness components following Baselga [33], the turnover component being the Simpson dissimilarity and the nestedness component the remainder, and each component was in turn related to elevational distance.
The analyses of richness and turnover were restricted to the 30 nights of 2021–2024, and the turnover analysis further to the 28 of those that yielded five or more species. The material collected between 2008 and 2014 was not determined to the same standard as the later collections, and those nights are systematically lower in elevation than the later ones (median 600 m against 1090 m, Mann–Whitney p = 0.003) as well as far poorer in species (3.6 against 13.5 species per night). Including them would confound elevation with the completeness of determination. They are retained in the checklist and in the occurrence dataset but excluded from the analyses.
All calculations were made in Python 3.12 with NumPy 2.4.4 and SciPy 1.17.1; the estimators and models were implemented directly from the published formulae rather than taken from a package. The code is provided as Supplementary File S2.
3. Results
3.1. Composition of the Fauna
The survey yielded 492 occurrence records of 1330 specimens, representing 161 species in 91 genera (Table 2). The two families are almost equally represented, with 78 species of Pyralidae and 83 of Crambidae. The Phycitinae are much the largest subfamily, with 61 species in 35 genera, followed by the Crambinae (23 species, 14 genera) and the Spilomelinae (22 species, 12 genera); the Scopariinae contribute 10 species in only two genera, and the Schoenobiinae a single species.
The catch is dominated by a small number of species. Udea ferrugalis alone accounts for 243 of the 1330 specimens (18.3%), followed by Endotricha flammealis (97), Metasia ophialis (81), Eudonia lacustrata (61) and Palpita vitrealis (46); the ten commonest species together account for 678 specimens (51.0%). At the other extreme, 44 species are known from a single specimen and 67 from a single locality.
3.2. New Records for Mersin Province
Eighty of the 161 species are reported here for the first time from Mersin Province (Table 2). The assessment rests on five sources: the national catalogue [1], checked species by species against the provincial range codes; the two annotated lists for the district of Anamur [11,12]; the updated distributional list of the Turkish Phycitinae [34]; an unpublished doctoral thesis on the Pyraloidea of Adana, Mersin and Osmaniye [10]; and the applied entomological literature, which the national catalogue does not always absorb.
The last two sources removed six species from the count that the catalogue alone would have left in it. Eight species absent from the 2018 catalogue had already been published from Anamur, three of them explicitly as new to the provincial fauna. Ectomyelois ceratoniae and Cryptoblabes gnidiella have been recorded from citrus and pomegranate orchards in the province by agricultural entomologists [2,3]. Four species — Angustalius malacellus, Metacrambus carectellus, Pediasia luteella and Udea prunalis — appear in the thesis of [10] but in no published source, and are retained as first published records with a note against each.
The new records are not evenly distributed among the subfamilies: 29 are Phycitinae and 16 Crambinae, together more than half the total. All eight species of Acrobasis and all four of Evergestis recorded here are new to the province. Thirty-seven of the eighty rest on a single record and are marked as such.
3.3. Nomenclature
Checking every name against GlobIZ altered 28 entries relative to the source material. Five species proved to belong to genera other than those under which they had been listed: Laodamia combustella (as Alophia), Chrysocramboides craterella (as Chrysocrambus), Ectomyelois ceratoniae (as Apomyelois), Myelopsis tetricella (as Episcythrastis) and Thopeutis cicatricella (as Friedlanderia). Pyrausta neglectalis Caradja, 1916 is treated in GlobIZ as a synonym of P. virginalis Duponchel, 1832, and the two entries were merged. The remaining changes concern misspellings, authorship, date and the use of parentheses. Both combinations are given in the checklist, because much of the regional literature uses the earlier ones.
Ten of the species were described from Anatolian type localities: Cadra delattinella (Akşehir), Elegia fallax (Amasya), Ephelis cruentalis (İzmir), Euclasta splendidalis (Asia Minor), Phycitodes inquinatella (Kahramanmaraş), Polyocha venosa (Asia Minor), Scotomera caesarealis (Kayseri), Taftania serratella (Mardin), Tegostoma lepidalis (Amasya) and Zophodiodes leucocostella (Amasya). Amasya accounts for three of the ten.
3.4. Distribution Along the Elevational Gradient
The number of species recorded rises with elevation across the four belts: 37 below 400 m, 55 between 401 and 800 m, 74 between 801 and 1200 m and 110 above 1200 m (Table 3). Sampling effort, however, also rises (12, 14, 11 and 17 nights; 8, 14, 8 and 15 localities), and a negative binomial model of the number of species per night against elevation and sampling month, fitted to the 30 nights of 2021–2024, gave no significant effect of elevation (β = 0.344, SE = 0.238, p = 0.149); adding the district as a term did not change this (β = 0.305, p = 0.211). The apparent increase in richness with elevation is therefore reported as an observation and is not supported as a tested result.
Compositional turnover gives a clearer signal. Across the 378 pairs of sampling events from the 28 nights analysed, the Sørensen dissimilarity increased with the elevational distance between the events (Spearman ρ = 0.187, p = 2.5 × 10⁻⁴). The effect is not attributable to season: dissimilarity was unrelated to the difference in sampling month (ρ = 0.076, p = 0.14), and controlling for month left the elevational correlation essentially unchanged (partial ρ = 0.178). Dissimilarity is high throughout, averaging 0.852, and did not differ between pairs within the same belt and pairs in different belts (0.847 against 0.855, Mann–Whitney p = 0.58), so that the turnover is gradual rather than organised into discrete belts (Figure 2).
Partitioning the total dissimilarity into its components shows that the difference between assemblages is almost entirely one of species replacement rather than of impoverishment. Of a mean total dissimilarity of 0.852, the turnover component accounts for 0.804 (94%) and the nestedness component for only 0.048 (6%). The two components behave oppositely along the gradient: the turnover component increases with elevational distance (ρ = 0.177, p = 5.5 × 10⁻⁴) while the nestedness component decreases (ρ = −0.135, p = 0.009). The fauna of the upper belts is therefore not a depauperate subset of the lowland fauna but a different assemblage.
Forty-six species were found only in the highest belt, against 17 confined to the 801–1200 m belt, 16 to the 401–800 m belt and 10 to the lowest; 72 species occur in more than one belt. The species confined to the upper belt include most of the specialised Phycitinae of dry karstic grassland, while the lowest belt, almost entirely under irrigated cultivation and urban expansion, holds mainly species of disturbed and cultivated ground. The proportions of the larger subfamilies also shift with elevation: the Phycitinae rise from 35% of the species in the lowest belt to 42% in the highest, while the Spilomelinae fall from 27% to 13%.
3.5. Completeness of the Inventory
Sixty-five of the 161 species were taken on only one of the 54 nights and 28 on two. Restricted to the 30 nights of 2021–2024, the Chao2 estimator gives 200 species against 146 observed, so that roughly three-quarters of the fauna likely to be present has been recorded (Figure 3). Applied to all 54 nights the estimator gives 235 against 161 observed, the inflation coming from the singletons contributed by the earlier, incompletely determined material. The rarefaction curve for the 24 nights of 2008–2014 flattens at 50 species, of which 31 are known from a single night; a proportion of singletons of 62% over 24 nights is not credible for a fauna of this kind and reflects incomplete determination rather than genuine rarity.
4. Discussion
4.1. the Scale of the New-Record Count
That so large a proportion of the list should be new to a province with a long collecting history reflects the distribution of that history rather than any peculiarity of the fauna. Most of the older material from Mersin comes from the coastal strip and from the Gülek pass on the old road over the Taurus, and the recent work concerns Anamur at the western end of the province. The intervening districts, including Erdemli and Mezitli, have been little collected, and the light-trap has been used in them hardly at all.
4.2. Comparison with the Pyraloidea of Köprülü Canyon
The only comparable survey from the Turkish Mediterranean is that of Şen and Akın [35], who worked the Köprülü Canyon National Park in Antalya Province with light traps between 2022 and 2024 and recorded 88 species from 24 localities and 1,018 specimens, between 127 and 1,459 m. The two studies are close enough in method and setting to be set side by side. The present survey covered 45 localities and a wider elevational range, 150 to 1,800 m, and produced 161 species from 1,330 specimens; forty-five species are common to both lists. The difference in species number reflects the number of localities and the length of the collecting period rather than any striking difference between the two faunas, and the two lists share the same subfamily structure, with the Phycitinae much the largest in each (61 species here, 44 at Köprülü Canyon).
Two points of contrast are worth stating. The first is favourable to the Antalya study: Şen and Akın dissected genitalia where external characters were insufficient, and were therefore able to report species of Ephestia, Epischnia, Phycitodes and Cadra without qualification, whereas the corresponding records here are provisional. The second concerns the state of provincial knowledge. Before their survey only 30 pyraloid species were on record from Antalya, a province of 20,000 square kilometres; 72 of their 88 species were new to it. The proportion here is lower, 80 of 161, but the two figures point the same way. Provincial lists for this superfamily in Türkiye rest on so little collecting that a single season of light-trapping in a previously unworked district can double them.
4.3. Species Described From Anatolia
Ten of the species recorded here carry Anatolian type localities, and the distribution of those localities is itself informative. Three are from Amasya, and the others from Akşehir, İzmir, Kahramanmaraş, Kayseri, Mardin and, in two cases, from “Asia Minor” without further specification. These are not centres of endemism but the places where nineteenth-century collectors worked, or through which they passed: Amasya was visited repeatedly by travelling naturalists and became, in effect, the type locality of a large part of the Anatolian microlepidoptera. The pattern reflects the itineraries of Staudinger, Mann, Lederer and their contemporaries rather than any biological concentration.
Two further species have type localities immediately beyond the Anatolian border, Laristania lydella in Georgia and Prochoristis crudalis and Glaucocharis euchromiella in Syria, and two subspecies of Acrobasis were described from Anatolian material: A. fallouella anatolica from Konya, Akşehir and İzmir, and A. consociella jessica from Kızılcahamam. The material reported here was not determined to subspecies, and these names are given for completeness rather than as records.
That a survey of two districts should recover ten species described from Anatolia is a measure of how thinly the country has been worked since. Four of the ten — Scotomera caesarealis, Taftania serratella, Tegostoma lepidalis and Zophodiodes leucocostella — are reported here for the first time from Mersin Province, and a fifth, Cadra delattinella, would be were it not among the species left provisional. Several of these are known from few localities and few specimens, and their type localities remain among the handful of places from which they have been reported.
4.4. Conservation
None of the 45 localities lies within a protected area. Neither Erdemli nor Mezitli contains a Wildlife Development Area or other reserve under the Turkish protected-area system, so that the whole of the fauna reported here was taken on unprotected land. The upper belt, which holds most of the specialised Phycitinae and the great majority of the species found only once, is under pressure from summer housing, road building and grazing, and the lowest belt is almost entirely converted to irrigated cultivation and urban expansion. The absence of any protected area in two districts that together span 150 to 1,800 m is worth stating plainly, because a fauna of this size cannot be assumed to persist without it.
4.5. Limitations
Identification. Genitalic dissection was not undertaken. Thirty species belong to genera that cannot be separated reliably on external characters and are treated as provisional; the grounds and the distribution of the effect among genera are set out in the Methods. Two further species are provisional on different grounds. Kemal et al. [12] describe Elegia feminina from Anamur and state that the specimen concerned had previously been identified as E. fallax on external similarity alone; the two records of fallax reported here were determined in the same way. The same authors describe their identification of Mecyna trinalis as temporary and note that the Taurus populations of the genus require examination of the genitalia and of genetic distances; the five records here come from the same range.
Sampling. Effort was not standardised. Collecting took place on 54 nights spread over sixteen years and nine seasons, with long gaps, and was concentrated in July and August. Only one locality was worked per night, and thirty-eight of the 45 localities were worked on a single night, five on two and two on three. The material from 2008–2014 was, moreover, not worked up as fully as the more recent collections, so that the early nights are represented by fewer species than the later ones. For these reasons the data are presented as a faunistic inventory and as an occurrence dataset, and no quantitative comparison is drawn between the two districts or between seasons. The consequences of this for the richness estimate are set out in Section 4.2.
5. Conclusions
The Pyraloidea of Erdemli and Mezitli comprise at least 161 species, eighty of them previously unrecorded from Mersin Province, and the estimators indicate that a quarter of the fauna remains to be found. The composition of the fauna changes gradually with elevation rather than in discrete belts, and the apparent increase in richness with height could not be separated from sampling effort. That so large a proportion of the list should be new to a province with a long collecting history reflects the distribution of that history rather than any peculiarity of the fauna: the districts between the coast and Anamur have simply not been worked with a light trap. Neither district contains a protected area, and the upper belt, which holds most of the specialised fauna and almost all the species found only once, is under pressure from summer housing, road building and grazing.
Supplementary Materials
The following supporting information can be downloaded at the website of this paper posted on Preprints.org: File S1, the occurrence dataset, 492 records formatted to the Darwin Core standard; File S2, the code used for the rarefaction, richness estimation and turnover analyses.
Author Contributions
Conceptualization, Y.H.; methodology, Y.H.; software, Y.H.; formal analysis, Y.H.; investigation, Y.H., E.K., A.K., S.A. and E.B.; resources, E.K., A.K., S.A. and E.B.; data curation, Y.H., E.K., A.K., S.A. and E.B.; writing—original draft preparation, Y.H.; writing—review and editing, E.K., A.K., S.A. and E.B.; visualization, Y.H.; supervision, Y.H.; project administration, Y.H.; funding acquisition, Y.H. All authors have read and agreed to the published version of the manuscript.
Funding
This research was supported in part by the Scientific Research Projects Unit of Mersin University (Project Numbers: 2021-1-TP2-4326, 2021-2-TP2-4521, 2022-1-TP2-4701, 2023-2-TP2-4962).
Institutional Review Board Statement
Not applicable.
Data Availability Statement
All occurrence records underlying the study are provided as Supplementary File S1, in Darwin Core format. The analysis code is provided as Supplementary File S2. Voucher specimens are deposited in the Entomological Research Laboratory (ENTOLAB), Department of Biology, Mersin University.
Acknowledgments
The authors thank Serdar Sönmez for preparing Figure 1. The fieldwork and the identification of the material were carried out at Mersin University, where all five authors were based at the time. During the preparation of this manuscript, the authors used Claude Opus 4.1 (Anthropic) for the purposes of drafting and editing the English text, compiling and checking the occurrence dataset, producing Figures 2 and 3, and writing the code used for the statistical analyses (File S2). All taxonomic decisions, identifications, verification against the primary literature and interpretation of the results are the authors' own. The authors have reviewed and edited the output and take full responsibility for the content of this publication.
Conflicts of Interest
The authors declare no conflicts of interest.
References
- Koçak, A.Ö.; Kemal, M. A Synonymous and Distributional List of the Species of the Lepidoptera of Turkey; Centre for Entomological Studies Ankara, Memoirs 8: Ankara, Türkiye, 2018; p. 489 pp. [Google Scholar]
- Öztürk, N.; Ölçülü, M.; Ulusoy, M.R. Adana ve Mersin ili turunçgil bahçelerinde harnup güvesi [Ectomyelois ceratoniae Zell. (Lepidoptera: Pyralidae)]’nin ergin popülasyon değişimi. Bitki Koruma Bülteni (In Turkish) 2011, 51, 347–358. [Google Scholar]
- Öztürk, N.; Ulusoy, M.R. Determination of adult population dynamics and generation number of honeydew moth, Cryptoblabes gnidiella Millière, 1867 (Lepidoptera: Pyralidae), in pomegranate orchards in the Eastern Mediterranean Region. Türk. Entomol. Derg. 2012, 36, 101–112. [Google Scholar]
- Elekçioğlu, N.Z. Adana’da Trabzon hurması bahçelerinde portakal güvesi [Cryptoblabes gnidiella Millière, 1867 (Lepidoptera: Pyralidae)]’nin popülasyon değişimi, zarar oranı ve mücadelesi. Çukurova Tarım Gıda Bilim. Derg. (In Turkish) 2019, 34, 149–160. [Google Scholar] [CrossRef]
- Sertkaya, E.; Akmeşe, V.; Atay, E. Türkiye’de mısırda yeni bir zararlı, Chilo partellus (Swinhoe) (Lepidoptera: Crambidae). Türk. Entomol. Bült. (In Turkish) 2014, 4, 197–200. [Google Scholar] [CrossRef]
- Kaçar, G.; Atay, E.; Koca, A.S.; Şahin, B. New distribution areas and identification characters of Loxostege sticticalis L. (Lepidoptera: Crambidae). Mustafa Kemal Univ. J. Agric. Sci. 2023, 28, 153–165. [Google Scholar] [CrossRef]
- Atay, E. Hatay İlinde Bulunan Pyraloidea (Lepidoptera) Faunası Üzerine Taksonomik-Sistematik Çalışmalar. MSc Thesis, (In Turkish) Mustafa Kemal University, Hatay, Türkiye, 2000. [Google Scholar]
- Aytekin, H.U.; Kütük, M. Gaziantep İli Crambidae (Lepidoptera: Pyraloidea) Faunasının Belirlenmesi. Kafkas Üniv. Fen. Bilim. Enst. Derg. (In Turkish) 2011, 4, 9–16. [Google Scholar]
- Akın, K. Mutki İlçesi (Bitlis) Pyralidae (Lepidoptera) Faunası ve Ekolojisi Üzerine Araştırmalar. PhD Thesis, (In Turkish) Van Yüzüncü Yıl University, Graduate School of Natural and Applied Sciences, Van, Türkiye, 2014. [Google Scholar]
- Atay, E. Adana, Mersin, Osmaniye İllerinde Bulunan Pyraloidea (Lepidoptera) Faunası Üzerine Taksonomik ve Sistematik Çalışmalar. PhD Thesis, (In Turkish) Çukurova University, Adana, Türkiye, 2005. [Google Scholar]
- Kemal, M.; Koçak, A.Ö. Annotated list of the moth fauna of Anamur district (İçel Prov., South Turkey), with descriptions of new species. Misc. Pap. Cent. Entomol. Stud. Ank. 2018, 167, 1–45. [Google Scholar]
- Kemal, M.; Kızıldağ, S.; Koçak, A.Ö. Annotated list of the Heterocera (Lepidoptera) of Anamur district (İçel Province, South Turkey) with description of a new species. Priamus 2020, 19, 1–72. [Google Scholar]
- Kılıç, A. Mersin İli Erdemli İlçesi Pyralidae (Lepidoptera) Familyası Üzerine Faunistik ve Taksonomik Araştırmalar. MSc Thesis, (In Turkish) Mersin University, Mersin, Türkiye, 2022. [Google Scholar]
- Kılıç, E. Mersin İli Erdemli İlçesi Crambidae (Lepidoptera) Familyası Üzerine Faunistik ve Taksonomik Araştırmalar. MSc Thesis, (In Turkish) Mersin University, Mersin, Türkiye, 2022. [Google Scholar]
- Atak, S. Mersin İli Mezitli İlçesi Crambidae (Lepidoptera) Familyası Üzerine Faunistik ve Taksonomik Araştırmalar. MSc Thesis, (In Turkish) Mersin University, Mersin, Türkiye, 2024. [Google Scholar]
- Bahçeci, E. Mersin İli Mezitli İlçesi Pyralidae (Lepidoptera) Familyası Üzerine Faunistik ve Taksonomik Araştırmalar. MSc Thesis, (In Turkish) Mersin University, Mersin, Türkiye, 2025. [Google Scholar]
- Atalay, İ. Vegetation Geography of Turkey; Ege Üniversitesi Basımevi: İzmir, Türkiye, 1994; p. 352 pp. [Google Scholar]
- Slamka, F. Pyraloidea of Europe. In Pyralinae, Galleriinae, Epipaschiinae, Cathariinae, Odontiinae; F. Slamka: Bratislava, Slovakia, 2006; Vol. 1, p. 138 pp. [Google Scholar]
- Slamka, F. Pyraloidea of Europe. In Crambinae and Schoenobiinae; F. Slamka: Bratislava, Slovakia, 2008; Vol. 2, p. 224 pp. [Google Scholar]
- Slamka, F. Pyraloidea of Europe. In Pyraustinae and Spilomelinae; F. Slamka: Bratislava, Slovakia, 2013; Vol. 3, p. 357 pp. [Google Scholar]
- Slamka, F. Pyraloidea of Europe. In Phycitinae, Part 1; F. Slamka: Bratislava, Slovakia, 2019; Vol. 4, p. 432 pp. [Google Scholar]
- Goater, B.; Nuss, M.; Speidel, W. Pyraloidea I (Crambidae: Acentropinae, Evergestinae, Heliothelinae, Schoenobiinae, Scopariinae). In Microlepidoptera of Europe; Huemer, P., Karsholt, O., Eds.; Apollo Books: Stenstrup, Denmark, 2005; Vol. 4, p. 304 pp. [Google Scholar]
- Nuss, M.; Landry, B.; Mally, R.; Vegliante, F.; Tränkner, A.; Bauer, F.; Hayden, J.; Segerer, A.; Schouten, R.; Li, H.; et al. Global Information System on Pyraloidea. Available online: www.pyraloidea.org (accessed on 10 July 2026).
- Agenjo, R. Las Pyrausta melanalis Caradja, 1916 y neglectalis Caradja, 1916 descritas de Cuenca, nuevas sinónimas, respectivamente, de Pyrausta purpuralis (Linneo, 1758) y Syllythria virginalis (Duponchel, 1831). Eos Rev. Esp. Entomol. (In Spanish) 1974, 50, 7–18. [Google Scholar]
- Fleischmann, M.; Van den Bossche, J.; Jordahl, K.; Richards, M.J.; McBride, J.; Wasserman, J.; Ward, B.; Wolf, L.J. GeoPandas: fundamental data structures for vector spatial data in Python. Comput. Environ. Urban Syst. 2026, 130, 102495. [Google Scholar] [CrossRef]
- Hunter, J.D. Matplotlib: a 2D graphics environment. Comput. Sci. Eng. 2007, 9, 90–95. [Google Scholar] [CrossRef]
- Harris, C.R.; Millman, K.J.; van der Walt, S.J.; Gommers, R.; Virtanen, P.; Cournapeau, D.; Wieser, E.; Taylor, J.; Berg, S.; Smith, N.J.; et al. Array programming with NumPy. Nature 2020, 585, 357–362. [Google Scholar] [CrossRef] [PubMed]
- McKinney, W. Data structures for statistical computing in Python. In Proceedings of the 9th Python in Science Conference; Austin, TX, USA, van der Walt, S., Millman, J., Eds.; 28 June–3 July 2010; pp. 56–61. [Google Scholar] [CrossRef]
- Harrower, M.; Brewer, C.A. ColorBrewer.org: an online tool for selecting colour schemes for maps. Cartogr. J. 2003, 40, 27–37. [Google Scholar] [CrossRef]
- Brewer, C.A.; Hatchard, G.W.; Harrower, M. ColorBrewer in print: a catalog of color schemes for maps. Cartogr. Geogr. Inf. Sci. 2003, 30, 5–32. [Google Scholar] [CrossRef]
- ttezer. Türkiye harita verisi: administrative boundary data for Türkiye. GitHub repository, 2026. Available online: https://github.com/ttezer/turkiye-harita-verisi (accessed on 3 September 2026).
- Chao, A. Estimating the population size for capture–recapture data with unequal catchability. Biometrics 1987, 43, 783–791. [Google Scholar] [CrossRef] [PubMed]
- Baselga, A. Partitioning the turnover and nestedness components of beta diversity. Glob. Ecol. Biogeogr. 2010, 19, 134–143. [Google Scholar] [CrossRef]
- Kemal, M.; Koçak, A.Ö. On the Phycitinae of Turkey: updated synonymic and distributional list of species (Lepidoptera) with some remarks. Priamus 2020, 18, 130–154. [Google Scholar]
- Şen, M.M.; Akın, K. Studies on the fauna of Pyraloidea (Lepidoptera) of Köprülü Canyon National Park (Antalya). Bitlis Eren Üniv. Fen. Bilim. Derg. 2025, 14, 1655–1671. [Google Scholar] [CrossRef]
Figure 1.
Sampling localities in the districts of Erdemli and Mezitli, Mersin Province, southern Türkiye. (a) Position of the study area (red outline) within Türkiye, on the southern flank of the central Taurus range; the three conventional subdivisions of the Taurus are indicated. (b) The 45 sampling localities, numbered as in Table 1 and coloured by elevational belt; the green frame marks the area enlarged in (c). (c) Enlargement of the eastern Mezitli cluster. Coordinates are on the WGS 84 datum, projected to UTM zone 36N. Boundary data from ttezer [31].
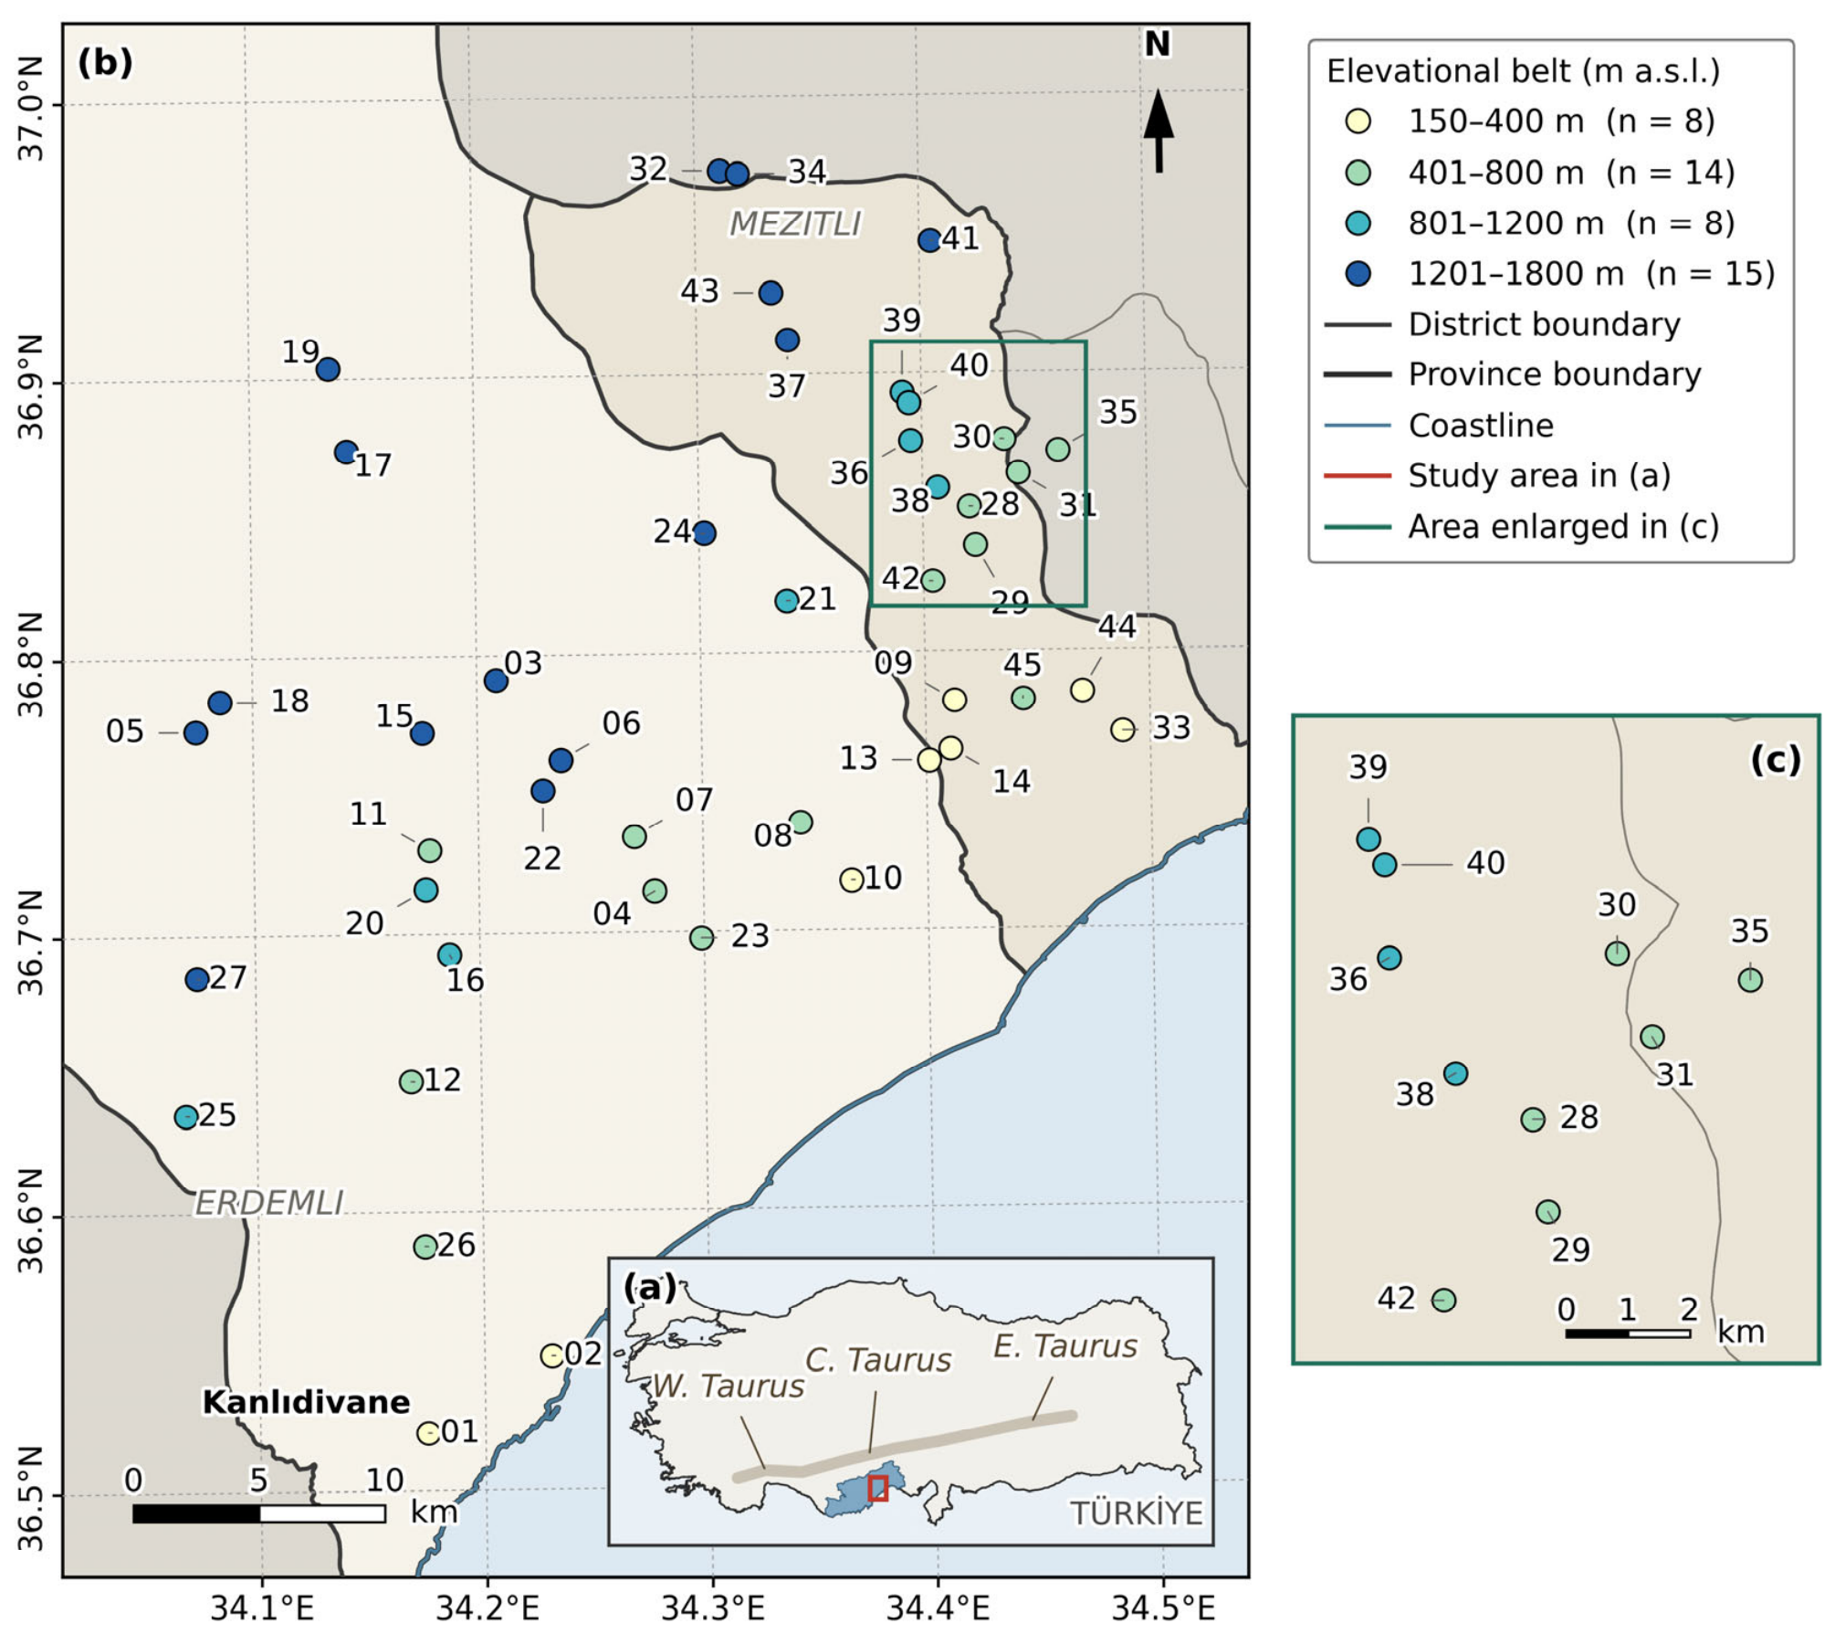
Figure 2.
Compositional turnover, from 378 pairs of the 28 sampling events analysed. (a) Sørensen dissimilarity against the elevational distance between events; the line is a least-squares fit. (b) The same against the difference in sampling month. (c) Dissimilarity within and between elevational belts. (d) Partition of the mean total dissimilarity into its turnover and nestedness components following Baselga [33]. Statistics are Spearman rank correlations in (a) and (b) and a Mann–Whitney test in (c).
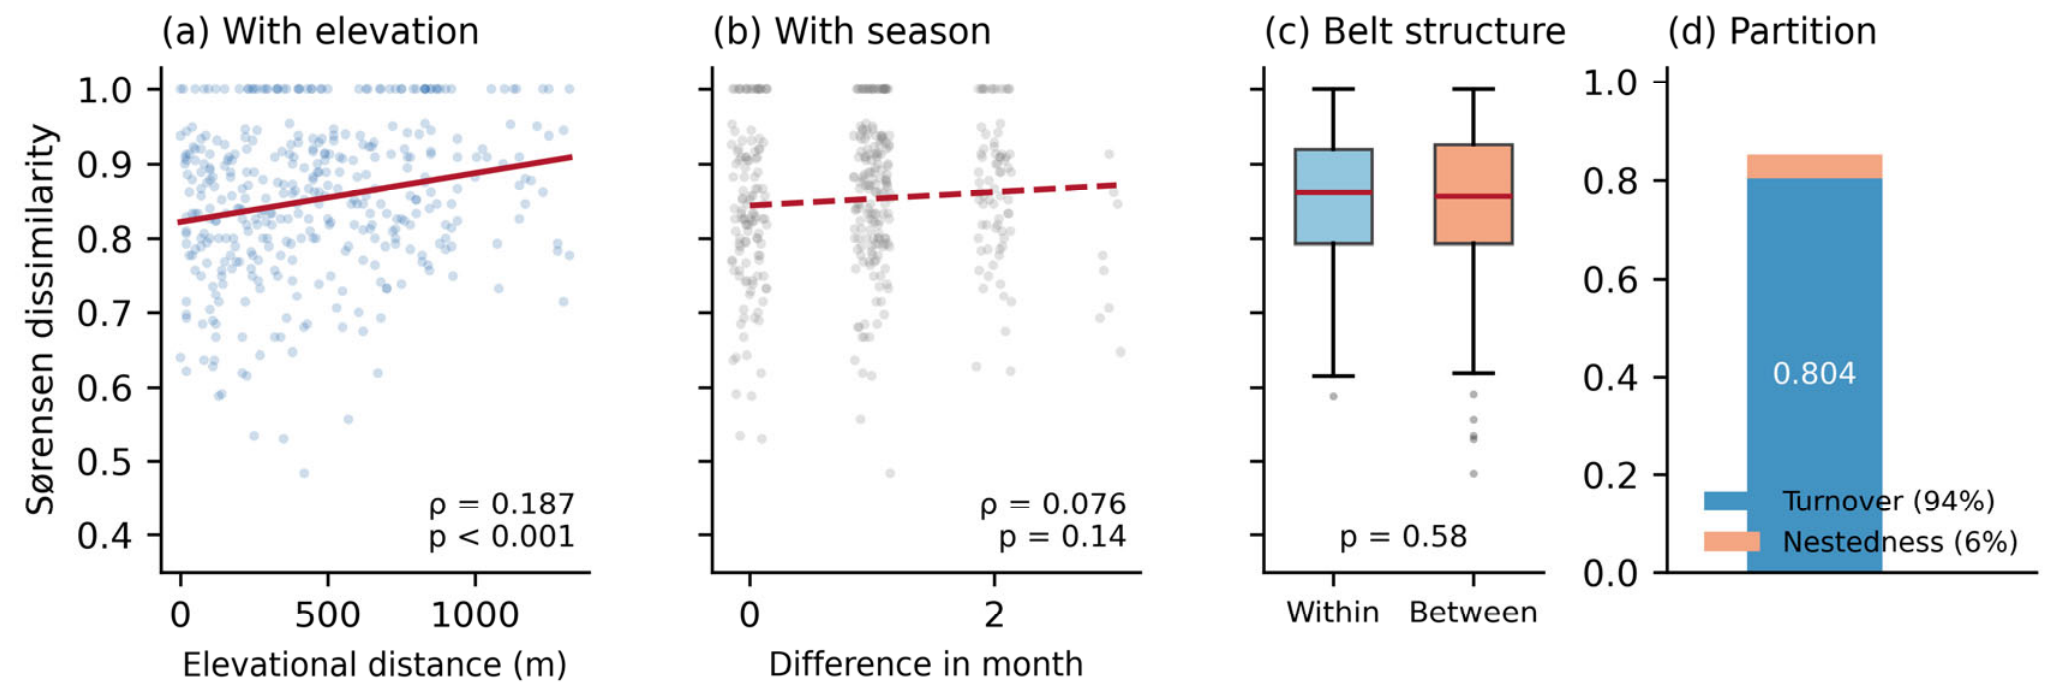
Figure 3.
Completeness of the Pyraloidea inventory. (a) Sample-based rarefaction curves for all 54 sampling nights and for the two collecting periods separately, with 95% confidence bands from 1000 randomisations of sample order. (b) Observed species richness and the incidence-based Chao2 estimate for the same three sets of nights, with the percentage of the estimated fauna recorded.
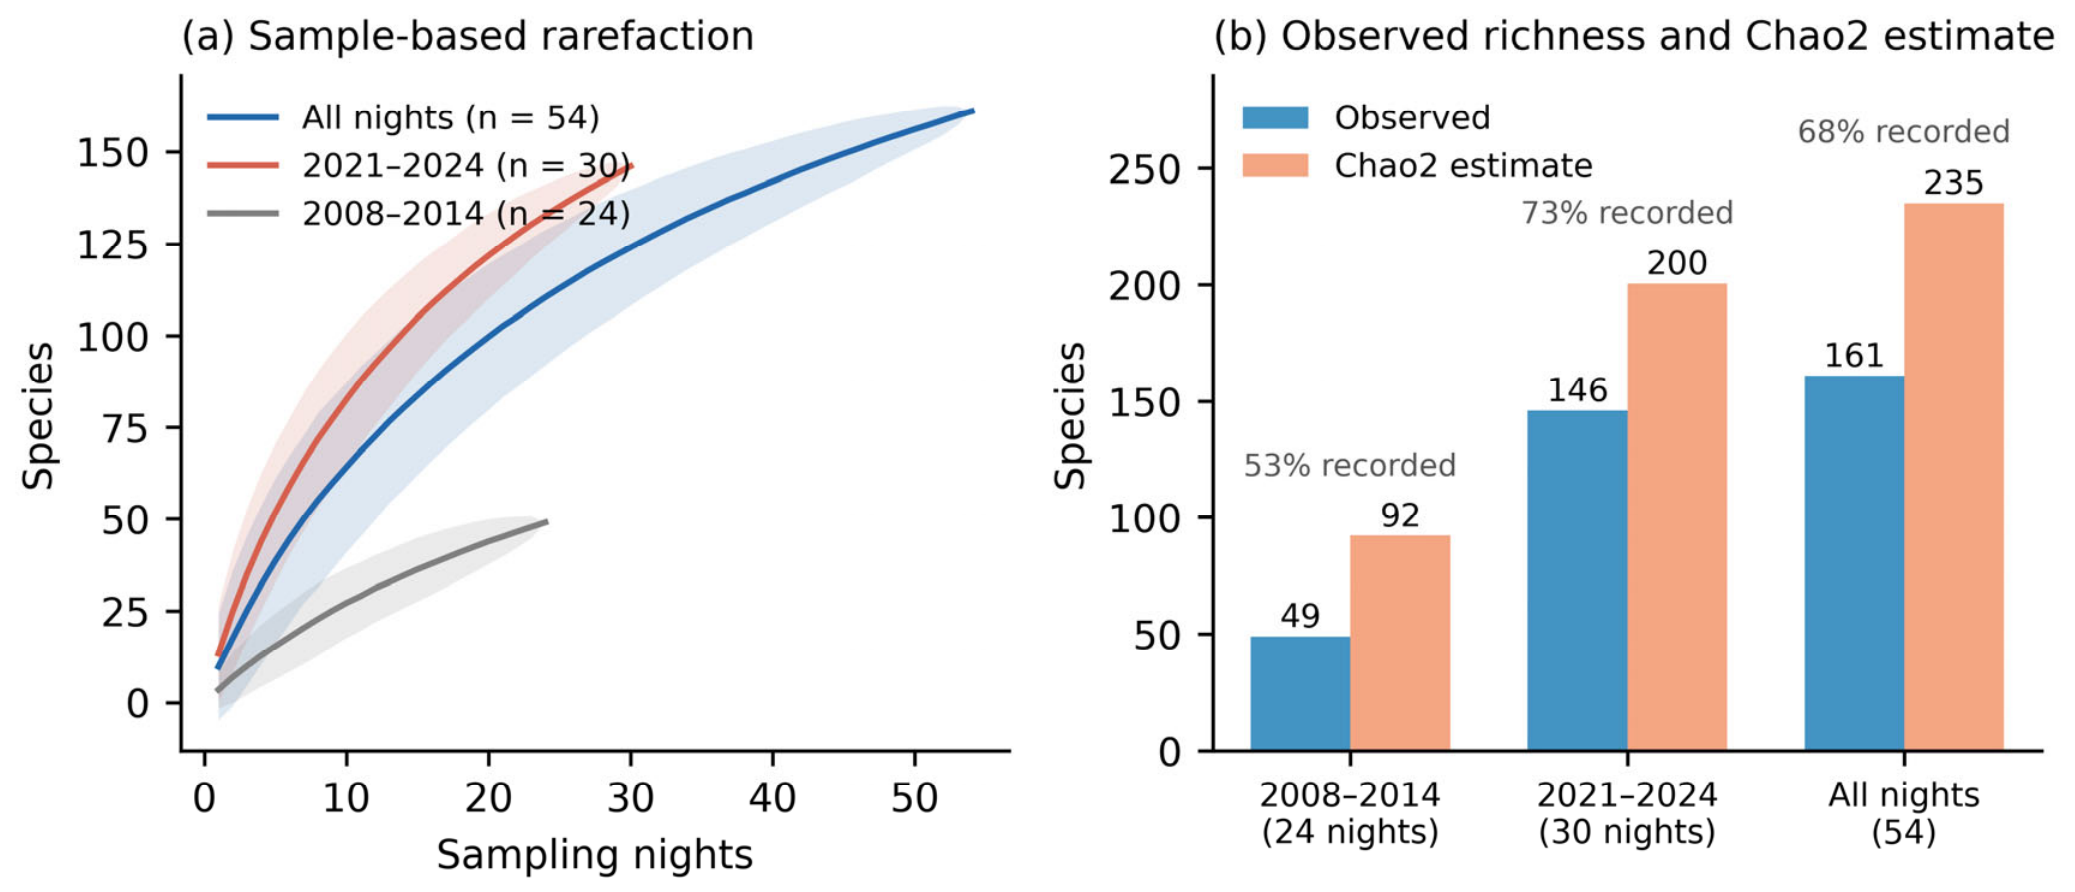

Table 1.
Sampling localities. Localities are numbered as in Figure 1. Coordinates are in decimal degrees on the WGS 84 datum. The coordinate uncertainty is derived from the spread of the sampling points combined within each locality (Section 2.5); elevations are given as a range where points at different elevations were combined.
| No. | District | Locality | Elevation (m) | Latitude (N) | Longitude (E) | Coordinate uncertainty (m) | No. of nights |
| 01 | Erdemli | Kanlıdivane | 250 | 36.52250 | 34.17444 | 850 | 2 |
| 02 | Erdemli | Limonlu | 300 | 36.54972 | 34.22972 | 250 | 1 |
| 03 | Erdemli | Hacıalanı S. | 1600 | 36.79306 | 34.20861 | 250 | 2 |
| 04 | Erdemli | Karahıdırlı güneyi | 500 | 36.71639 | 34.27806 | 250 | 1 |
| 05 | Erdemli | Güzeloluk güneyi | 1320–1380 | 36.77528 | 34.07444 | 250 | 2 |
| 06 | Erdemli | Kafeli | 1300 | 36.76389 | 34.23694 | 250 | 1 |
| 07 | Erdemli | Karahıdırlı N. | 700 | 36.73611 | 34.26917 | 250 | 1 |
| 08 | Erdemli | Sıraç güneyi | 600 | 36.74056 | 34.34333 | 250 | 1 |
| 09 | Erdemli | Yeşil Mahalle | 250 | 36.78389 | 34.41278 | 250 | 1 |
| 10 | Erdemli | Elvanlı | 250 | 36.71944 | 34.36583 | 250 | 1 |
| 11 | Erdemli | Koramşalı | 800 | 36.73194 | 34.17806 | 250 | 1 |
| 12 | Erdemli | Çerçili | 760 | 36.64889 | 34.16861 | 250 | 1 |
| 13 | Erdemli | Doğusandal güneyi | 250 | 36.76222 | 34.40111 | 250 | 1 |
| 14 | Erdemli | Doğusandal | 300 | 36.76639 | 34.41083 | 250 | 1 |
| 15 | Erdemli | Çerçili kuzeyi | 1300 | 36.77417 | 34.17528 | 250 | 1 |
| 16 | Erdemli | Arslanlı | 1180 | 36.69444 | 34.18639 | 250 | 1 |
| 17 | Erdemli | Sorgun | 1590 | 36.87583 | 34.14306 | 250 | 1 |
| 18 | Erdemli | Güzeloluk batısı | 1320 | 36.78611 | 34.08528 | 250 | 1 |
| 19 | Erdemli | Toros Köyü | 1700 | 36.90556 | 34.13528 | 250 | 1 |
| 20 | Erdemli | Kösereli kuzeyi | 1200 | 36.71778 | 34.17611 | 250 | 1 |
| 21 | Erdemli | Sinap kuzeydoğusu | 1056 | 36.82028 | 34.33861 | 250 | 1 |
| 22 | Erdemli | Çamlı kuzeyi | 1250 | 36.75306 | 34.22889 | 250 | 1 |
| 23 | Erdemli | Yeşildere kuzeyi | 470 | 36.69944 | 34.29861 | 250 | 1 |
| 24 | Erdemli | Şahna batısı | 1300 | 36.84500 | 34.30222 | 250 | 1 |
| 25 | Erdemli | Tapureli güneyi | 1040 | 36.63722 | 34.06833 | 250 | 1 |
| 26 | Erdemli | Batısandal | 450 | 36.58944 | 34.17389 | 250 | 1 |
| 27 | Erdemli | Alibeyli doğusu | 1230 | 36.68667 | 34.07389 | 250 | 1 |
| 28 | Mezitli | Kuzucu | 750 | 36.85333 | 34.42056 | 250 | 1 |
| 29 | Mezitli | Kuzucubelen | 600 | 36.83972 | 34.42306 | 250 | 1 |
| 30 | Mezitli | Doğançay S. | 600 | 36.87750 | 34.43639 | 250 | 1 |
| 31 | Mezitli | Uzunkaş | 700 | 36.86528 | 34.44250 | 250 | 1 |
| 32 | Mezitli | Fındıkpınarı, Durnaz (1800 m) | 1800 | 36.97528 | 34.31111 | 250 | 1 |
| 33 | Mezitli | Kuyuluk | 150–200 | 36.77204 | 34.48759 | 800 | 3 |
| 34 | Mezitli | Fındıkpınarı, Durnaz Mevkii (1700 m) | 1700 | 36.97417 | 34.31917 | 250 | 1 |
| 35 | Mezitli | Doğançay W | 420 | 36.87333 | 34.46056 | 250 | 1 |
| 36 | Mezitli | Akarca N. | 855–870 | 36.87736 | 34.39486 | 250 | 2 |
| 37 | Mezitli | Bozön Güzlesi N | 1475 | 36.91417 | 34.34056 | 250 | 1 |
| 38 | Mezitli | Akarca NW | 870 | 36.86028 | 34.40667 | 250 | 1 |
| 39 | Mezitli | Fındıkpınarı S | 970 | 36.89472 | 34.39139 | 250 | 1 |
| 40 | Mezitli | Fındıkpınarı SE | 1070–1100 | 36.89093 | 34.39426 | 250 | 3 |
| 41 | Mezitli | Demirışık | 1220 | 36.94917 | 34.40472 | 250 | 1 |
| 42 | Mezitli | Kuzucu W | 760 | 36.82694 | 34.40389 | 250 | 1 |
| 43 | Mezitli | Bozön Güzlesi NW | 1550 | 36.93111 | 34.33333 | 250 | 1 |
| 44 | Mezitli | Cemilli E | 380–400 | 36.78681 | 34.46986 | 250 | 2 |
| 45 | Mezitli | Cemilli W | 550 | 36.78417 | 34.44333 | 250 | 1 |
Table 2.
Annotated checklist. Species are arranged by family and subfamily and alphabetically within each subfamily. “Locality numbers” refers to the localities of Table 1; “No. of localities” is the number of those localities; “Records” is the number of occurrence records and “Specimens” the number of individuals. * new record for Mersin Province; a known from a single record; b reported by [10] in an unpublished thesis but not in any published source. † provisional identification, genitalic examination required; ‡ provisional on other grounds (Section 2.4).
| No. | Species | New | Prov. | Locality numbers | No. of localities | Records | Specimens | Elevation (m) |
| Pyralidae: Galleriinae | ||||||||
| 1 | Aphomia cephalonica (Stainton, 1866) | *a | 26 | 1 | 1 | 1 | 450 | |
| 2 | Aphomia sociella (Linnaeus, 1758) | *a | 24 | 1 | 1 | 1 | 1300 | |
| 3 | Lamoria anella ([Denis & Schiffermüller], 1775) | * | 9, 10, 19, 35, 39, 40, 42, 44, 45 | 9 | 10 | 15 | 250–1700 | |
| 4 | Lamoria zelleri (Joannis, 1932) | * | 9, 11, 16, 26, 34, 35 | 6 | 6 | 7 | 250–1700 | |
| Pyralidae: Pyralinae | ||||||||
| 5 | Aglossa caprealis (Hübner, 1809) | * | 5, 15, 17, 20, 35 | 5 | 5 | 5 | 420–1590 | |
| 6 | Endotricha flammealis ([Denis & Schiffermüller], 1775) | 5, 10, 14, 15, 16, 26, 37, 38, 39, 40, 41, 42, 44, 45 | 14 | 15 | 97 | 250–1475 | ||
| 7 | Hypotia corticalis ([Denis & Schiffermüller], 1775) | 26, 35 | 2 | 2 | 2 | 420–450 | ||
| 8 | Hypsopygia costalis (Fabricius, 1775) | 2, 25, 27 | 3 | 3 | 3 | 300–1230 | ||
| 9 | Hypsopygia rubidalis ([Denis & Schiffermüller], 1775) | * | 5, 16, 20 | 3 | 3 | 5 | 1180–1320 | |
| 10 | Loryma egregialis (Herrich-Schäffer, 1838) | 39 | 1 | 1 | 1 | 970 | ||
| 11 | Pyralis kacheticalis (Christoph, 1893) | 17, 19, 25, 40 | 4 | 4 | 4 | 1040–1700 | ||
| 12 | Pyralis regalis [Denis & Schiffermüller], 1775 | 5, 17, 18, 20, 22, 24, 27, 42 | 8 | 8 | 16 | 760–1590 | ||
| 13 | Scotomera caesarealis (Ragonot, 1891) | *a | 44 | 1 | 1 | 1 | 400 | |
| 14 | Stemmatophora brunnealis (Treitschke, 1829) | *a | 43 | 1 | 1 | 1 | 1550 | |
| 15 | Stemmatophora combustalis (Fischer von Röslerstamm, 1842) | *a | 23 | 1 | 1 | 1 | 470 | |
| 16 | Synaphe punctalis (Fabricius, 1775) | 5, 37 | 2 | 2 | 2 | 1380–1475 | ||
| 17 | Tretopteryx pertusalis (Geyer, 1832) | 1, 9 | 2 | 3 | 3 | 250 | ||
| Pyralidae: Phycitinae | ||||||||
| 18 | Acrobasis centunculella (Mann, 1859) | * | 16, 27 | 2 | 2 | 3 | 1180–1230 | |
| 19 | Acrobasis consociella (Hübner, 1813) | * | 35, 39, 40, 42, 44, 45 | 6 | 6 | 14 | 400–1100 | |
| 20 | Acrobasis fallouella (Ragonot, 1871) | * | 5, 9, 16, 20, 25, 26, 27, 40, 42, 44 | 10 | 10 | 13 | 250–1320 | |
| 21 | Acrobasis glaucella Staudinger, 1859 | * | 15, 20, 34, 35, 39, 40, 41, 44, 45 | 9 | 10 | 33 | 380–1700 | |
| 22 | Acrobasis legatea (Haworth, 1811) | 22 | 1 | 1 | 1 | 1250 | ||
| 23 | Acrobasis obliqua (Zeller, 1847) | *a | 25 | 1 | 1 | 3 | 1040 | |
| 24 | Acrobasis repandana (Fabricius, 1798) | *a | 5 | 1 | 1 | 1 | 1320 | |
| 25 | Acrobasis suavella (Zincken, 1818) | * | 5, 15, 25, 41 | 4 | 4 | 5 | 1040–1320 | |
| 26 | Acrobasis tumidana ([Denis & Schiffermüller], 1775) | *a | 4 | 1 | 1 | 1 | 500 | |
| 27 | Anerastia lotella (Hübner, 1813) | *a | 26 | 1 | 1 | 1 | 450 | |
| 28 | Bradyrrhoa gilveolella (Treitschke, 1833) | *a | 34 | 1 | 1 | 1 | 1700 | |
| 29 | Cadra cautella (Walker, 1863) | † | 23, 44, 45 | 3 | 3 | 4 | 400–550 | |
| 30 | Cadra delattinella Roesler, 1965 | † | 34, 42 | 2 | 2 | 2 | 760–1700 | |
| 31 | Cadra figulilella (Gregson, 1871) | † | 27 | 1 | 1 | 1 | 1230 | |
| 32 | Cadra furcatella (Herrich-Schäffer, 1849) | † | 27 | 1 | 1 | 1 | 1230 | |
| 33 | Cryptoblabes gnidiella (Millière, 1867) | 17 | 1 | 1 | 2 | 1590 | ||
| 34 | Delplanqueia dilutella ([Denis & Schiffermüller], 1775) | † | 17 | 1 | 1 | 1 | 1590 | |
| 35 | Denticera divisella (Duponchel, 1842) | 1, 3, 5, 15, 16, 17, 18, 19, 27, 35, 39, 40, 44 | 13 | 16 | 25 | 250–1700 | ||
| 36 | Dioryctria abietella ([Denis & Schiffermüller], 1775) | * | 5, 11, 12, 15, 17, 18, 19, 21 | 8 | 9 | 11 | 760–1700 | |
| 37 | Dioryctria mendacella (Staudinger, 1859) | 4, 5, 7, 8, 15, 18, 21, 37, 38, 40 | 10 | 10 | 17 | 500–1475 | ||
| 38 | Dioryctria simplicella Heinemann, 1865 | *a | 32 | 1 | 1 | 1 | 1800 | |
| 39 | Dioryctria sylvestrella (Ratzeburg, 1840) | * | 17, 34 | 2 | 2 | 2 | 1590–1700 | |
| 40 | Ectomyelois ceratoniae (Zeller, 1839) | 36, 39 | 2 | 2 | 2 | 855–970 | ||
| 41 | Elegia fallax (Staudinger, 1881) | ‡ | 15, 40 | 2 | 2 | 2 | 1080–1300 | |
| 42 | Ematheudes punctellus (Treitschke, 1833) | 16, 18, 40, 41 | 4 | 4 | 7 | 1080–1320 | ||
| 43 | Ephestia elutella (Hübner, 1796) | † | 40, 44, 45 | 3 | 3 | 4 | 400–1080 | |
| 44 | Ephestia kuehniella Zeller, 1879 | † | 5 | 1 | 1 | 2 | 1320 | |
| 45 | Epischnia adultella Zeller, 1848 | † | 10 | 1 | 1 | 1 | 250 | |
| 46 | Epischnia cretaciella Mann, 1869 | † | 10, 12, 17 | 3 | 3 | 6 | 250–1590 | |
| 47 | Epischnia prodromella (Hübner, 1799) | † | 6, 17, 39 | 3 | 3 | 3 | 970–1590 | |
| 48 | Etiella zinckenella (Treitschke, 1832) | 3, 17, 34, 39, 40 | 5 | 5 | 10 | 970–1700 | ||
| 49 | Euzophera bigella (Zeller, 1848) | 16, 17, 18 | 3 | 3 | 4 | 1180–1590 | ||
| 50 | Gymnancyla canella ([Denis & Schiffermüller], 1775) | 10, 17, 19 | 3 | 3 | 3 | 250–1700 | ||
| 51 | Homoeosoma nimbella (Duponchel, [1837]) | † | 19 | 1 | 1 | 1 | 1700 | |
| 52 | Homoeosoma sinuella (Fabricius, 1794) | † | 19, 20 | 2 | 2 | 2 | 1200–1700 | |
| 53 | Hypsotropa limbella Zeller, 1848 | * | 17, 35, 36, 38, 39, 41, 44, 45 | 8 | 8 | 26 | 400–1590 | |
| 54 | Laodamia combustella (Herrich-Schäffer, [1855]) | * | 5, 16, 40 | 3 | 3 | 4 | 1080–1320 | |
| 55 | Laristania lydella (Lederer, 1865) | *a | 17 | 1 | 1 | 1 | 1590 | |
| 56 | Laristania nevadensis (Rebel, 1910) | *a | 32 | 1 | 1 | 3 | 1800 | |
| 57 | Lymphia chalybella (Eversmann, 1844) | *a | 40 | 1 | 1 | 1 | 1080 | |
| 58 | Myelois multiforella Ragonot, 1893 | *a | 37 | 1 | 1 | 1 | 1475 | |
| 59 | Myelopsis tetricella ([Denis & Schiffermüller], 1775) | *a | 17 | 1 | 1 | 1 | 1590 | |
| 60 | Pempelia alpigenella (Duponchel, 1836) | † | 5, 17, 34 | 3 | 3 | 15 | 1320–1700 | |
| 61 | Pempelia palumbella ([Denis & Schiffermüller], 1775) | † | 5, 18, 19, 35, 44 | 5 | 5 | 7 | 400–1700 | |
| 62 | Pempeliella sororiella (Zeller, 1839) | † | 25 | 1 | 1 | 1 | 1040 | |
| 63 | Phycita poteriella (Zeller, 1846) | *a | 15 | 1 | 1 | 1 | 1300 | |
| 64 | Phycita roborella ([Denis & Schiffermüller], 1775) | * | 5, 27, 36, 40 | 4 | 4 | 5 | 855–1320 | |
| 65 | Phycita torrenti Agenjo, 1962 | * | 36, 40 | 2 | 2 | 2 | 855–1100 | |
| 66 | Phycitodes albatella (Ragonot, 1887) | † | 21, 38, 40, 41 | 4 | 4 | 5 | 870–1220 | |
| 67 | Phycitodes binaevella (Hübner, 1813) | † | 17, 18, 44 | 3 | 3 | 5 | 380–1590 | |
| 68 | Phycitodes inquinatella (Ragonot, 1887) | † | 40 | 1 | 2 | 4 | 1080–1100 | |
| 69 | Phycitodes lacteella (Rothschild, 1915) | † | 34, 36, 39, 40, 43 | 5 | 6 | 28 | 855–1700 | |
| 70 | Phycitodes saxicola (Vaughan, 1870) | † | 39, 40, 41, 42 | 4 | 5 | 29 | 760–1220 | |
| 71 | Pima leucoloma (Herrich-Schäffer, [1849]) | 17, 40 | 2 | 2 | 2 | 1100–1590 | ||
| 72 | Polyocha venosa (Zeller, 1847) | 40 | 1 | 2 | 2 | 1080–1100 | ||
| 73 | Psorosa mediterranella Amsel, 1954 | *a | 5 | 1 | 1 | 2 | 1320 | |
| 74 | Pyla fusca (Haworth, 1811) | * | 5, 21 | 2 | 2 | 3 | 1056–1320 | |
| 75 | Sciota hostilis (Stephens, 1834) | * | 5, 18 | 2 | 2 | 4 | 1320 | |
| 76 | Selagia spadicella (Hübner, 1796) | *a | 18 | 1 | 1 | 2 | 1320 | |
| 77 | Taftania serratella (Ragonot, 1893) | * | 38, 39 | 2 | 2 | 5 | 870–970 | |
| 78 | Zophodiodes leucocostella Ragonot, 1887 | * | 39, 42, 44, 45 | 4 | 4 | 5 | 400–970 | |
| Crambidae: Scopariinae | ||||||||
| 79 | Eudonia angustea (J. Curtis, 1827) | † | 34 | 1 | 1 | 1 | 1700 | |
| 80 | Eudonia delunella (Stainton, 1849) | † | 15, 21, 27 | 3 | 3 | 6 | 1056–1300 | |
| 81 | Eudonia lacustrata (Panzer, 1804) | † | 17, 21, 22, 23, 25, 27, 34, 36, 37, 43 | 10 | 10 | 61 | 470–1700 | |
| 82 | Eudonia mercurella (Linnaeus, 1758) | † | 5, 16, 17, 18, 32 | 5 | 5 | 6 | 1180–1800 | |
| 83 | Eudonia phaeoleuca (Zeller, 1846) | † | 23, 25, 26 | 3 | 3 | 3 | 450–1040 | |
| 84 | Scoparia ambigualis (Treitschke, 1829) | † | 12 | 1 | 1 | 2 | 760 | |
| 85 | Scoparia basistrigalis Knaggs, 1866 | † | 22, 37 | 2 | 2 | 5 | 1250–1475 | |
| 86 | Scoparia ingratella (Zeller, 1846) | † | 22 | 1 | 1 | 3 | 1250 | |
| 87 | Scoparia pyralella ([Denis & Schiffermüller], 1775) | † | 5, 6, 16, 17, 22, 27 | 6 | 6 | 7 | 1180–1590 | |
| 88 | Scoparia subfusca Haworth, 1811 | † | 21 | 1 | 1 | 2 | 1056 | |
| Crambidae: Crambinae | ||||||||
| 89 | Agriphila geniculea (Haworth, 1811) | *a | 8 | 1 | 1 | 2 | 600 | |
| 90 | Agriphila inquinatella ([Denis & Schiffermüller], 1775) | 2 | 1 | 1 | 2 | 300 | ||
| 91 | Agriphila straminella ([Denis & Schiffermüller], 1775) | *a | 16 | 1 | 1 | 4 | 1180 | |
| 92 | Agriphila tolli (Błeszyński, 1952) | * | 7, 8, 23 | 3 | 3 | 4 | 470–700 | |
| 93 | Ancylolomia palpella ([Denis & Schiffermüller], 1775) | 6, 8, 45 | 3 | 3 | 6 | 550–1300 | ||
| 94 | Angustalius malacellus (Duponchel, 1836) | *ab | 39 | 1 | 1 | 1 | 970 | |
| 95 | Catoptria acutangulellus (Herrich-Schäffer, 1847) | * | 37, 43 | 2 | 2 | 4 | 1475–1550 | |
| 96 | Catoptria falsella ([Denis & Schiffermüller], 1775) | * | 3, 5 | 2 | 2 | 7 | 1380–1600 | |
| 97 | Catoptria mytilella (Hübner, [1805]) | *a | 18 | 1 | 1 | 4 | 1320 | |
| 98 | Catoptria pinella (Linnaeus, 1758) | 3, 39, 41 | 3 | 3 | 3 | 970–1600 | ||
| 99 | Chrysocramboides craterella (Scopoli, 1763) | 12, 17, 18, 24, 27, 40 | 6 | 6 | 14 | 760–1590 | ||
| 100 | Chrysocrambus linetella (Fabricius, 1781) | 17, 34 | 2 | 2 | 3 | 1590–1700 | ||
| 101 | Euchromius anapiellus (Zeller, 1847) | *a | 44 | 1 | 1 | 1 | 400 | |
| 102 | Euchromius bella (Hübner, 1796) | 26, 44 | 2 | 2 | 6 | 400–450 | ||
| 103 | Euchromius rayatella (Amsel, 1949) | * | 5, 23, 26 | 3 | 3 | 6 | 450–1320 | |
| 104 | Euchromius superbellus (Zeller, 1849) | * | 20, 26, 27, 40, 44 | 5 | 5 | 13 | 400–1230 | |
| 105 | Glaucocharis euchromiella (Ragonot, 1895) | 18, 20, 21 | 3 | 3 | 6 | 1056–1320 | ||
| 106 | Mesocrambus candiellus (Herrich-Schäffer, 1848) | * | 36, 39 | 2 | 2 | 3 | 855–970 | |
| 107 | Metacrambus carectellus (Zeller, 1847) | *b | 17, 19, 36 | 3 | 3 | 7 | 855–1700 | |
| 108 | Neocrambus wolfschlaegeri (Schawerda, 1937) | *a | 17 | 1 | 1 | 1 | 1590 | |
| 109 | Pediasia luteella ([Denis & Schiffermüller], 1775) | *ab | 18 | 1 | 1 | 1 | 1320 | |
| 110 | Pseudobissetia terrestrellus (Christoph, 1885) | *a | 35 | 1 | 1 | 1 | 420 | |
| 111 | Thopeutis cicatricella (Hübner, [1824]) | *a | 26 | 1 | 1 | 1 | 450 | |
| Crambidae: Schoenobiinae | ||||||||
| 112 | Donacaula niloticus (Zeller, 1867) | * | 18, 36, 39, 41 | 4 | 4 | 5 | 855–1320 | |
| Crambidae: Glaphyriinae | ||||||||
| 113 | Hyperlais dulcinalis (Treitschke, 1835) | *a | 40 | 1 | 1 | 9 | 1080 | |
| 114 | Prochoristis crudalis (Lederer, 1863) | *a | 44 | 1 | 1 | 2 | 380 | |
| Crambidae: Odontiinae | ||||||||
| 115 | Cynaeda dentalis ([Denis & Schiffermüller], 1775) | * | 4, 18, 34, 35, 36 | 5 | 5 | 11 | 420–1700 | |
| 116 | Ephelis cruentalis (Geyer, 1832) | 17, 18, 24, 28, 31, 32, 34, 37, 40 | 9 | 9 | 14 | 700–1800 | ||
| 117 | Tegostoma lepidalis (Herrich-Schäffer, 1851) | * | 15, 16, 17 | 3 | 3 | 3 | 1180–1590 | |
| Crambidae: Evergestinae | ||||||||
| 118 | Evergestis aenealis ([Denis & Schiffermüller], 1775) | *a | 17 | 1 | 1 | 5 | 1590 | |
| 119 | Evergestis mundalis (Guenée, 1854) | * | 17, 19 | 2 | 2 | 14 | 1590–1700 | |
| 120 | Evergestis pallidata (Hufnagel, 1767) | * | 3, 6 | 2 | 3 | 4 | 1300–1600 | |
| 121 | Evergestis subfuscalis (Staudinger, 1870) | * | 5, 19 | 2 | 2 | 3 | 1320–1700 | |
| Crambidae: Pyraustinae | ||||||||
| 122 | Achyra nudalis (Hübner, 1796) | 4 | 1 | 1 | 1 | 500 | ||
| 123 | Anania perlucidalis (Hübner, [1809]) | *a | 34 | 1 | 1 | 1 | 1700 | |
| 124 | Ecpyrrhorrhoe diffusalis (Guenée, 1854) | * | 16, 20, 35 | 3 | 3 | 4 | 420–1200 | |
| 125 | Euclasta splendidalis (Herrich-Schäffer, 1848) | 21 | 1 | 1 | 2 | 1056 | ||
| 126 | Loxostege sticticalis (Linnaeus, 1761) | * | 27, 34, 36 | 3 | 3 | 4 | 855–1700 | |
| 127 | Loxostege turbidalis (Treitschke, 1829) | *a | 17 | 1 | 1 | 1 | 1590 | |
| 128 | Paracorsia repandalis ([Denis & Schiffermüller], 1775) | *a | 35 | 1 | 1 | 1 | 420 | |
| 129 | Pyrausta aurata (Scopoli, 1763) | 10, 23, 24 | 3 | 3 | 3 | 250–1300 | ||
| 130 | Pyrausta castalis Treitschke, 1829 | * | 9, 21, 34 | 3 | 3 | 10 | 250–1700 | |
| 131 | Pyrausta despicata (Scopoli, 1763) | 4, 18, 27 | 3 | 3 | 3 | 500–1320 | ||
| 132 | Pyrausta falcatalis Guenée, 1854 | 23 | 1 | 1 | 2 | 470 | ||
| 133 | Pyrausta limbopunctalis (Herrich-Schäffer, 1849) | 22 | 1 | 1 | 1 | 1250 | ||
| 134 | Pyrausta ostrinalis (Hübner, 1796) | * | 3, 6, 22 | 3 | 3 | 5 | 1250–1600 | |
| 135 | Pyrausta purpuralis (Linnaeus, 1758) | 17, 18 | 2 | 2 | 4 | 1320–1590 | ||
| 136 | Pyrausta sanguinalis (Linnaeus, 1767) | 24 | 1 | 1 | 3 | 1300 | ||
| 137 | Pyrausta virginalis Duponchel, 1832 | * | 9, 23, 34, 40, 43, 44 | 6 | 7 | 8 | 250–1700 | |
| 138 | Sitochroa verticalis (Linnaeus, 1758) | 42 | 1 | 1 | 1 | 760 | ||
| 139 | Uresiphita gilvata (Fabricius, 1794) | 38 | 1 | 1 | 1 | 870 | ||
| Crambidae: Spilomelinae | ||||||||
| 140 | Antigastra catalaunalis (Duponchel, 1833) | 44 | 1 | 1 | 3 | 400 | ||
| 141 | Dolicharthria punctalis ([Denis & Schiffermüller], 1775) | 9, 24 | 2 | 2 | 9 | 250–1300 | ||
| 142 | Duponchelia fovealis Zeller, 1847 | 13 | 1 | 1 | 1 | 250 | ||
| 143 | Hydriris ornatalis (Duponchel, 1832) | 36 | 1 | 1 | 1 | 855 | ||
| 144 | Mecyna auralis (Peyerimhoff, 1872) | *a | 34 | 1 | 1 | 1 | 1700 | |
| 145 | Mecyna flavalis ([Denis & Schiffermüller], 1775) | * | 5, 16, 18, 32 | 4 | 4 | 7 | 1180–1800 | |
| 146 | Mecyna trinalis ([Denis & Schiffermüller], 1775) | ‡ | 5, 16, 20, 21, 37 | 5 | 5 | 15 | 1056–1475 | |
| 147 | Metasia carnealis (Treitschke, 1829) | 12, 18, 35 | 3 | 3 | 7 | 420–1320 | ||
| 148 | Metasia ophialis (Treitschke, 1829) | * | 5, 12, 17, 18, 19, 20, 21, 22, 34, 36, 37, 39, 40, 44, 45 | 15 | 15 | 81 | 400–1700 | |
| 149 | Nomophila noctuella ([Denis & Schiffermüller], 1775) | 9, 11, 12, 13, 22, 37, 40 | 7 | 7 | 34 | 250–1475 | ||
| 150 | Palpita vitrealis (Rossi, 1794) | 1, 5, 10, 11, 12, 25, 33, 34, 35, 40, 42, 44 | 12 | 15 | 46 | 150–1700 | ||
| 151 | Patania balteata (Fabricius, 1798) | 28 | 1 | 1 | 1 | 750 | ||
| 152 | Spoladea recurvalis (Fabricius, 1775) | 2, 33 | 2 | 2 | 6 | 150–300 | ||
| 153 | Synclera traducalis (Zeller, 1852) | 35 | 1 | 1 | 1 | 420 | ||
| 154 | Udea bipunctalis (Herrich-Schäffer, 1848) | * | 6, 8, 26, 29, 30 | 5 | 5 | 13 | 450–1300 | |
| 155 | Udea ferrugalis (Hübner, 1796) | 1, 9, 10, 15, 16, 22, 25, 37, 38, 39, 40, 41, 43, 44, 45 | 15 | 15 | 243 | 250–1550 | ||
| 156 | Udea fulvalis (Hübner, 1809) | * | 35, 36 | 2 | 2 | 2 | 420–855 | |
| 157 | Udea institalis (Hübner, 1819) | *a | 22 | 1 | 1 | 1 | 1250 | |
| 158 | Udea languidalis (Eversmann, 1842) | 37 | 1 | 1 | 1 | 1475 | ||
| 159 | Udea nebulalis (Hübner, 1796) | *a | 10 | 1 | 1 | 5 | 250 | |
| 160 | Udea numeralis (Hübner, 1796) | * | 5, 22 | 2 | 2 | 2 | 1250–1320 | |
| 161 | Udea prunalis ([Denis & Schiffermüller], 1775) | *b | 9, 24, 27 | 3 | 3 | 10 | 250–1300 | |
Table 3.
Distribution among elevational belts. Sampling effort is given as the number of localities and the number of sampling nights falling within each belt. “Exclusive species” is the number recorded in that belt only; 72 species occur in more than one belt. The last column gives the number of species of Pyralidae and of Crambidae.
| Elevational belt (m a.s.l.) | Localities | Nights | Species | Exclusive species | Pyralidae / Crambidae |
| 150–400 | 8 | 12 | 37 | 10 | 19 / 18 |
| 401–800 | 14 | 14 | 55 | 16 | 24 / 31 |
| 801–1200 | 8 | 11 | 74 | 17 | 41 / 33 |
| 1201–1800 | 15 | 17 | 110 | 46 | 57 / 53 |
| Total | 45 | 54 | 161 | 89 | 78 / 83 |
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.
Copyright: This open access article is published under a Creative Commons CC BY 4.0 license, which permit the free download, distribution, and reuse, provided that the author and preprint are cited in any reuse.