
Submitted:
08 September 2026
Posted:
09 September 2026
You are already at the latest version
Abstract
This review examines how eusociality reshapes breeding strategies in Apis mellifera and why honeybee colony phenotypes should be interpreted within a population-based framework. Rather than treating colonies as isolated breeding entities, we argue that interconnected populations of colonies represent the most relevant evolutionary scale for honeybee improvement, because genetic variation is continuously generated, exchanged, and filtered across colonies through reproduction, environmental pressures, and selection. The review first examines the genetic mechanisms that structure colony and population diversity. It then considers how non-genetic factors such as nutrition, landscape, disease pressure, management practices, and temporal variability shape colony phenotypes and constrain experimental repeatability, trait interpretation, and breeding evaluation. Together, these dimensions support a Genotype × Environment × Time (G×E×T) framework in honeybees that challenges breeding concepts largely derived from conventional livestock improvement programmes. From this perspective, breeding strategies grounded in population genetics, population-based mass selection, and conservation-oriented management are more consistent with honeybee biology than breeding frameworks derived from individually selected livestock species. Excessive reliance on a limited number of elite lineages may increase introgression, reduce effective population size, erode local adaptation, and weaken long-term adaptive potential. Acknowledging honeybee biological specificities, this review proposes a framework that reconciles conservation and breeding through a gradient of human selection intensity, ranging from protected conservation populations to managed hybridisation zones. Consequently, this review suggests solutions to reconcile conservation to breeding resulting in complementation of maintaining long-term evolution potential while assuring colony productivity.
Keywords:
Apis mellifera
; honeybee breeding
; population genetics
; mass selection
; genotype-by-environment interaction
; phenotyping
; genetic diversity
; local adaptation
; conservation
; adaptive potential
1. Introduction
In conventional agricultural species, phenotypic evaluation is predominantly centred on direct productivity metrics and economic performance at the individual level, with genetic progress achieved through controlled mating, pedigree tracking, and trait-based selective breeding [1]. In contrast, Apis mellifera occupies a unique position in animal agriculture: its biological and economic performance arises from a eusocial organisation in which reproductive asymmetry, division of labour, and distributed behavioural specialisation generate traits at the colony level. This superorganism structure limits the direct transposition of breeding frameworks developed for individually selected livestock species.
Consequently, the phenotype of a honeybee colony cannot be interpreted as the expression of a single genotype. Instead, colony phenotypes emerge from interactions among genetically diverse individuals, environmental conditions, and temporal dynamics operating simultaneously within the superorganism.
By examining the biological consequences of eusociality in honeybees, this review argues that colony phenotypes must be interpreted within a broader population-based framework. We show how the mechanisms generating and maintaining genetic diversity within and among colonies shape phenotypic variation, influence adaptation, and ultimately affect breeding outcomes. Building on these foundations, we propose that population-based mass selection and conservation-oriented approaches may be more consistent with honeybee biology than breeding strategies centred on a limited number of elite lineages.
Within a single apiary, substantial phenotypic variation is typically observed among colonies. Even colonies originating from the same maternal lineage often exhibit markedly different developmental trajectories, productivity, behaviour, and survival. Understanding the origin of this variation is fundamental because it forms the biological basis upon which both natural and artificial selection operate.
1.1. Intrinsic Mechanisms Generating Genetic Diversity in Apis mellifera (Section 2, Section 3 and Section 4)
Honeybee colony consists of thousands of genetically diverse individuals with varying degrees of relatedness, belonging to different developmental stages and age cohorts, and exposed to heterogeneous environmental conditions. Phenotypic variation among honeybee colonies is not merely the consequence of environmental noise but arises from biological mechanisms intrinsic to Apis mellifera that continuously generate and maintain genetic diversity. These mechanisms operate at multiple biological scales, from inheritance and mating systems to colony reproduction and population dynamics (Box 1).
| Box 1. Major biological mechanisms promoting genetic diversity in Apis mellifera. |
|
In addition to these genetic mechanisms, environmental conditions and beekeeping practices contribute substantially to phenotypic variation among colonies. Colony location, landscape composition, resource availability, climate, disease pressure, and management practices can all influence colony development, behaviour, productivity, and survival. Because these factors often interact, their individual effects are difficult to isolate experimentally, and colonies exposed to seemingly similar conditions may nevertheless exhibit markedly different phenotypes.
Time represents a third fundamental dimension shaping honeybee phenotypes. At the genetic level, temporal processes include development from egg to adult age-related polyethism, and changes in colony demographic structure. At the environmental level, temporal variation encompasses fluctuations in resource availability, pathogen pressure, climate, and seasonal colony dynamics. The interaction of genetic variation, environmental heterogeneity, and temporal dynamics generates a highly complex phenotypic system. This complexity supports a G×E×T framework in which time is as fundamental as genotype and environment in shaping honeybee colony phenotypes. Consequently, both genetic and environmental effects vary through time, making colony phenotypes inherently dynamic rather than fixed attributes of stable biological entities.
Section 2 and Section 3, and Section 4 examine these three dimensions separately. Section 2 focuses on the biological mechanisms that generate and redistribute genetic diversity, Section 3 examines environmental factors, nutrition, disease pressure, management practices, and their genotype-by-environment interactions (GEI) as drivers of phenotypic variation, and Section 4 explores how temporal dynamics interact with both genotype and environment to influence colony performance over time.
1.2. Consequences for Phenotyping and Breeding Frameworks (Section 5 and Section 6)
Unlike most livestock species, honeybee colonies are dynamic entities whose composition, organisation, and performance change continuously through time. Consequently, phenotypic measurements obtained at a single biological level or during a limited period may provide only a partial representation of colony phenotype.
These characteristics complicate the estimation of genetic value and breeding index that challenge the direct application of breeding frameworks developed for individually selected animals.
Accordingly, Section 5 and Section 6 argue that the biological characteristics of honeybees, together with the G×E×T framework developed throughout this review, naturally lead to a population-based perspective for phenotyping, selection, and management. Section 5 examines colony phenotypes as emergent outcomes of interacting genetic, environmental, and temporal factors, and discusses the resulting limitations and challenges associated with phenotyping, trait interpretation, and standardisation. Building on these considerations, Section 6 then explores how these insights support adaptive breeding and conservation frameworks in which populations are managed under different intensities of human selection, ranging from sanctuary populations exposed primarily to natural selection to innovation and hybridisation populations subjected to increasingly directed breeding objectives.
2. Genetic Drivers of Phenotypic Variation
2.1. High Rate of Recombination in Apis mellifera
Recombination during meiosis reshuffles genetic material through exchanges between homologous chromosomes, generating new allelic combinations. In most animals, recombination is limited—typically one or two chiasmata per chromosome pair—but recombination rate (RR) varies widely across taxa [26]. In A. mellifera, RR reaches extreme values unmatched among metazoans, making recombination a major biological driver of phenotypic variation.
2.1.1. Comparative Recombination Rate
The honeybee genome (~250 Mb; n = 16 chromosomes) exhibits RR estimates ranging from 19 cM/Mb [3] to 37 cM/Mb [4]. These values are an order of magnitude higher than in related or similarly sized genomes, including: Bombus terrestris: 4.4 cM/Mb [27], Average Hymenoptera: 7.12 ± 5.13 cM/Mb [27], Diptera: 1.03 ± 1.14 cM/Mb, Coleoptera: 2.48 ± 1.31 cM/Mb.
2.1.2. Genomic Distribution
Recombination hotspots are distributed across the honeybee genome, with rates reaching 143 cM/Mb in 125-kb windows [3], 197.7 cM/Mb in 200-kb windows [4], corresponding to ~5.7 crossovers per chromosome pair per meiosis. Chromosomes 1, 2, and 6 contain the highest density of recombination hot regions. Genome-wide analyses reveal strong correlations between RR and GC content, nucleotide diversity, gene density and copy number variation [4,29]. In addition to crossovers, non-crossing gene conversion events occur approximately 30× more often than crossovers [30], further contributing to GC-biased transmission of alleles [5].
2.2. The Csd Gene Mechanism Promotes Heterozygosity at the Sex Locus
Sex determination in A. mellifera. follows a complementary sex determination (csd) system, in which heterozygosity at the sex locus produces females, whereas hemizygosity (haploidy) or homozygosity (diploidy) produces males [31,32]. This system confers honeybees a distinctive genetic structure: viable males are haploid and derive from unfertilized eggs, while diploid male larvae—produced when a queen mates with a genetically related drone—are eliminated by workers during early development [6]. Consequently, the csd mechanism exerts strong selective pressure for high allelic diversity and avoidance of inbreeding, both of which contribute to overall genetic variation at the colony and population levels.
2.2.1. Haplodiploidy and Pedigree Structure
Because drones develop from unfertilized eggs, they carry a haploid genome identical to that of their mother’s gametes. Early apicultural geneticists (Newell 1915; summarized by [33]) referred to drones as “flying gametes” rather than members of a new generation. Modern interpretations of honeybee genealogies [34,35] consequently treat only females as generational units, underscoring the atypical logic of inheritance in haplodiploids. From a genetic perspective, queens therefore contribute directly to both female and male lineages, as drones originate from unfertilised eggs and represent expressed maternal gametes.
2.2.2. Consequences of Sex-Locus Homozygosity: “Shot Brood”
When queens mate with related drones—common under instrumental insemination with same-mother males—approximately 50% of fertilized eggs become homozygous at the csd locus and develop into diploid males [36,37]. Workers recognize and remove these larvae, resulting in the characteristic “shot brood” or “shotgun brood” pattern. This brood loss dramatically reduces colony performance and constitutes a major risk in closed breeding systems.
2.2.3. Molecular Architecture of the Sex Locus
The honeybee csd locus, located near the telomeric region of chromosome 8 [32,38], was mapped by [39] and cloned by positional cloning [6]. The csd gene encodes an SR-type protein with an N-terminal RS domain, a hypervariable region, rich in Asn/Tyr repeats, a C-terminal proline-rich domain.
This structural variability is central to allelic specificity. The csd protein is homologous to Drosophila Transformer (Tra), a key regulator of sex determination. Heteroallelic csd combinations trigger female development through female-specific splicing of the feminizer (fem) transcript, which subsequently regulates downstream sex-determination processes together with Transformer-2 (tra2) [40,41].
2.2.4. High Allelic Diversity at the Csd Locus
Allelic richness at the csd locus is exceptionally high. Early estimates reported 53–87 alleles in surveyed populations and extrapolated a worldwide diversity of approximately 116–145 alleles [42]. Subsequent studies have suggested that global csd diversity may be substantially higher than these initial estimates [43].
2.3. Enhanced Diversity Carried by the Drones Laid by the Workers
2.3.1. Drone Genetic Origins
In honeybees, drones originate from unfertilized haploid eggs and therefore carry only the genome of their mother (Figure 1). Typically, most drones in a queenright colony are produced by the queen. Depending on season and colony conditions, queens may generate up to 20,000 drones per year [44], although lower values such as 4,830 drones have also been reported [45].
Workers can also lay haploid eggs, although in queenright colonies this occurs at extremely low frequencies (≈ 0.12% of drones; [45]). However, in queenless colonies —particularly when there is no potential for requeening— worker ovary activation becomes common. Under such circumstances, a large cohort of workers develops functional ovaries, while others provide brood care, allowing the colony to rear up to 6,000 worker-origin drones [44]. Worker policing collapses in such colonies, enabling worker-laid eggs to develop.
The evolutionary logic of this system is straightforward: in a colony that has lost its queen and cannot replace her, the only remaining opportunity for genetic transmission is through the production of drones by workers. These workers transmit not only their own maternal genome but also the paternal genome inherited from drones that had previously mated the queen. Worker reproduction therefore preserves, to some extent, the genetic legacy of the dead queen and her mates. Because drones from queenless colonies derive from numerous workers belonging to different patrilines, they incorporate the recombination during queen oogenesis and the recombination in multiple workers originating from distinct patrilines (Figure 2).
As a result, the genetic diversity of drones produced by worker-laying colonies can exceed that of drones laid exclusively by a single queen. This genomic diversity has population-level consequences, especially during the mating season when such drones join DCAs (Figure 3).
2.3.2. Fitness and Fertility of Drones
Whether drones produced by queens and workers differ in fitness remains unresolved. Drone fertility, expressed primarily as sperm quantity and quality, is strongly influenced by developmental and nutritional conditions.
Queen-laid drones typically emerge slightly heavier than worker-laid drones (≈17% heavier at emergence; [46]), yet these differences diminish over time. Studies under semi-arid conditions similarly found that queen-derived drones had greater fertility than worker-derived drones [47].
Other studies contradict these findings. For instance, worker-derived drones may receive better larval care in queenless colonies [48]. They may be larger and carry more spermatozoa [49]. Egg size from worker-laid eggs is significantly larger (up to +22% volume; [50]), suggesting modified provisioning.
Nutritional limitation experiments yielded mixed results. Several studies suggested that pollen deprivation after emergence does not significantly affect male fecundity or sperm production [51,52,53], implying that male sexual maturation is largely completed during pupation.
Overall, sperm counts range from 3.6 to 12 million per drone [54], and drone body size positively correlates with sperm number [55]. The conflicting findings underline that environmental factors and colony status influence drone quality more strongly than their maternal origin.
Despite these uncertainties, one conclusion is robust: drones have undergone strong sexual selection [51] and are highly specialized for a single biological function—mating once, after which they die.
2.4. Multiple Mating as a Factor of Genetic Diversity Within the Colony and Between Colonies
Honeybee reproductive biology is structured to avoid inbreeding and maximize genetic diversity [11]. Polyandry, DCAs, and asynchronous sexual maturation of queens and drones all contribute to this diversity.
2.4.1. Differential Sexual Development Timing
Drone development to full sexual maturity takes approximately 36 days, whereas queens reach sexual maturity in about 22 days [56]. Virgin queens arise under different colony contexts (swarming, supersedure, or emergency replacement), and drone production is regulated by workers, environmental cues, and colony-level demographic needs. These asynchronous developmental trajectories reduce the likelihood that a virgin queen will mate with drones from her own colony.
2.4.2. Aerial Mating Limits Inbreeding
Queens fly to DCAs to mate in the air, ensuring they do not mate with drones from their own colony. Queens typically fly to more distant DCA, whereas drones preferentially fly to the nearest one [17]. This spatial behaviour ensures natural outcrossing at a landscape scale.
2.4.3. The DCA Organisation
DCAs are stable locations hosting large numbers of drones often reaching around 10,000 individuals [57]. Genetic analyses have shown that drones at a single DCA can originate from hundreds of surrounding colonies, with at least 243 colonies identified in one study [11]. Drones can fly up to 5 km and frequently drift between colonies, although many remain faithful to their natal hive [58]. DCAs therefore represent genetic melting points where drones from many colonies mix. The effective sex ratio in the mating environment is highly skewed (1 queen : 1,000–2,000 drones).
2.4.4. Number of Mating and Effective Paternity
Polyandry is one of the most distinctive reproductive characteristics of A. mellifera and a major generator of intracolony genetic diversity. Most queens mate with 12–14 drones on average, with reported minima of six and maxima of 26 [59]. Other studies have documented even higher mating frequencies under certain environmental conditions [60,61,62] (See Table 1 for an exhaustive chronological review of estimates of the number of drones mating with honey bee queens). These multiple matings have profound consequences for the representation of patrilines and effective paternity within the colony.
During the mating flight, a queen accumulates 100–200 million spermatozoa in her reproductive tract [63]. However, only a small proportion is ultimately stored: approximately 5 million spermatozoa are transferred to the spermatheca, after about 90% of the ejaculate has been expelled [17]. Sperm stored in the spermatheca can remain viable for years, although quality declines with queen age [64]. During the fertilisation of an individual oocyte, queens release on average approximately two spermatozoa from the spermatheca, although this number can range from 1 to >400 depending on queen age and physiological condition [65].
Whether sperm from different drones mix homogeneously in the spermatheca remains an unresolved question. Some studies support the idea of sperm clumping or stratification of patrilines [17], whereas others find no evidence of patriline bias and advocate for a fully mixed sperm pool [14,66]. Both mixing and clumping studies typically analyse one or very few queens and may capture only part of the temporal dynamics of sperm homogenisation. Early work using morphological mutants suggested that patriline proportions vary over time, albeit without consistent suppression or dominance of particular subfamilies [12].
A queen may lay up to 1.5 million fertilised eggs during her lifetime [65]. However, the concept of effective paternity—the number of drones whose sperm is equally and consistently represented among the queen’s offspring—is considerably more complex than the raw mating number. Classical estimates assume equal sperm mixing and equal representation of patrilines [67]. Recent molecular studies, however, challenge this assumption. Cryptic patrilines have been detected in colonies [68], and behavioural mechanisms such as kin recognition or biased brood care may influence larval survival and adult representation of subfamilies. This raises the possibility that some patrilines may be under-represented or transient within colonies.
In addition, drones themselves contribute variable numbers of spermatozoa (ranging from 3.6 to 12 million per drone; [54]), and drone fertility is influenced by environmental factors, larval nutrition, and colony status. Thus, the relative contribution of drones to the queen’s stored sperm depends not only on the number of mates but also on drone sperm quality. However, current evidence suggests minimal intra-spermathecal sperm competition [13], although the precise dynamics of sperm use still require further investigation.
These uncertainties have significant implications for colony phenotyping. If the genetic composition of worker cohorts changes through time —as a result of patriline turnover, non-random sperm use, or differential subfamily survival— then the colony itself becomes a genetically dynamic unit, not a static one. This temporal genetic fluidity complicates the assessment of colony-level traits and challenges breeding strategies that implicitly assume stable patriline representation.
Overall, the number of mating drones, the quantity and quality of sperm stored, and the pattern of sperm utilisation collectively determine effective paternity, shaping intracolony genetic architecture and influencing behavioural diversity, disease resilience, and colony performance. Beyond increasing intracolonial diversity, polyandry profoundly modifies the genetic architecture of the colony itself. The following sections examine how multiple mating generates colonies composed of interacting genetic subfamilies and why this complexity has major consequences for phenotyping and breeding.
2.5. Implication of Multiple Mating
2.5.1. The Colony as a Genetic Mosaic
Intracolony genetic diversity in A. mellifera arises primarily from the combination of two fundamental biological mechanisms: extremely high meiotic recombination during queen oogenesis and extreme polyandry, whereby a virgin queen mates with numerous drones during mating flights. Together, these processes generate colonies composed of genetically heterogeneous worker populations structured into multiple subfamilies (patrilines) [13,19,34].
To fully understand the genetic architecture of a honeybee colony, two hierarchical levels of paternal structure must be distinguished (Supplementary Table 1). First, workers sired by the same drone share an identical paternal haploid genome while differing in their maternally recombined haplotypes, forming a “supersister” group [34]. Second, because drones are haploid and transmit direct gametic representations of their mother queen’s genome, mating at DCAs also connects colonies through multiple queen-derived genetic lineages originating from the surrounding population [35]. Consequently, a virgin queen mates not only with multiple individual drones but indirectly with genetic material originating from numerous colonies across the landscape.
The resulting colony integrates several layers of relatedness generated by recombination, polyandry, and population-level mating processes. Rather than a collection of genetically equivalent individuals, the honeybee colony functions as a true genetic mosaic composed of multiple interacting patrilines. Many colony-level traits cannot be reduced to single genotypes or individual phenotypes, but emerge from interactions among genetically diverse subfamilies within the superorganism. This genetic mosaic creates a complex hierarchy of genetic relationships among colony members, which forms the basis of colony organisation and social evolution.
2.5.2. Genetic Relatedness Within Mosaic Colony
The genetic architecture of a honeybee colony differs radically from that of diploid, monogamous organisms. Relatedness varies asymmetrically among colony members due to haplodiploidy and polyandry.
Due to the combined effects of haplodiploidy and polyandry, genetic relatedness varies substantially among colony members. Workers belonging to the same patriline (supersisters) share an identical paternal genome and are related by r = 0.75, whereas workers originating from different patrilines (half-sisters) are related by only r = 0.25 [34,69]. Consequently, a honeybee colony is not a genetically homogeneous entity but a structured assemblage of overlapping genetic subfamilies connected through different degrees of relatedness.
Several complementary coefficients have been proposed to describe genetic relationships in haplodiploid societies, including kinship coefficients, Wright’s relatedness coefficients, and directional genetic transmission coefficients [34,70]. Together, these metrics illustrate the unusual relatedness structure generated by haplodiploidy, extreme polyandry, and asymmetric genome transmission (Supplementary Table 2).
This hierarchical genetic structure has important biological consequences. By creating genetically differentiated worker groups within the same colony, polyandry increases intracolonial genetic diversity while maintaining social cohesion through shared maternity. Colony organisation therefore emerges from interactions among individuals that are neither genetically identical nor genetically unrelated, but occupy intermediate and variable positions within a complex network of kinship relationships [71,72,73]. Beyond its evolutionary significance, this relatedness structure provides the genetic foundation upon which behavioural specialisation, division of labour, social immunity, and other emergent colony-level traits are expressed. The coexistence of multiple related but genetically distinct subfamilies creates the conditions under which genetic diversity can influence colony function, ultimately linking intracolonial genetic structure to colony-level phenotypes.
2.5.3. From Genetic Diversity to Functional Heterogeneity
The uneven relatedness structure generated by haplodiploidy and polyandry has profound consequences for colony organisation and function. Genomic, transcriptomic, and behavioural studies further demonstrate that worker responses and task allocation vary among patrilines [71,74,75]. Workers belonging to different patrilines differ in behavioural tendencies, developmental trajectories, disease resistance, survivorship, learning ability, and task allocation.
Consequently, intracolonial genetic diversity creates a heterogeneous workforce in which genetic subfamilies contribute differently to colony activities. Workers from different patrilines may differ in behavioural tendencies, developmental trajectories, learning ability, disease susceptibility, physiological responses, longevity, and responsiveness to environmental conditions. This functional heterogeneity increases the range of phenotypes expressed within the colony, potentially enhancing colony flexibility and resilience under variable environmental conditions.
This diversity has also stimulated longstanding questions regarding kin recognition and nepotism. Because workers belonging to the same patriline are more closely related to one another than to workers from different patrilines, it has been proposed that workers may preferentially direct cooperative behaviours towards closer relatives, thereby increasing their inclusive fitness [76,77]. However, support for nepotistic behaviour remains limited and controversial. While some studies have reported evidence consistent with kin discrimination, others failed to detect significant preferential treatment of close relatives [78,79]. Overall, colony-level cooperation appears to largely override individual kin preferences. Nevertheless, this debate highlights the importance of relatedness structure in shaping social interactions within colonies.
Beyond generating functional heterogeneity, the coexistence of multiple genetically distinct patrilines raises a more fundamental question: how should the genotype of a honeybee colony itself be defined?
2.5.4. What Is the Genotype of a Colony?
The concept of colony genotype in A. mellifera differs fundamentally from that of classical diploid organisms. In most animals, genotype can be represented by the genome of a single individual. In honeybees, however, the colony consists of thousands of genetically distinct individuals belonging to multiple patrilines and interacting within a social environment. Consequently, the genotype of a colony cannot be represented by a single genome, including that of the queen.
A useful conceptual distinction can therefore be made between the realised colony genotype and the potential colony genotype.
At any given time, the realised colony genotype may be viewed as the genetic composition of all living individuals constituting the superorganism:
where:
- is the queen genotype,
- is the set of worker genotypes present at time ,
- denotes the union of genotypes constituting the colony at time t.
One particularly remarkable aspect of honeybee reproductive biology is that the potential genetic repertoire of a colony is largely determined shortly after the queen’s mating flights. During this brief period, the queen acquires and stores sperm from multiple drones, creating a reservoir of paternal genomes that may contribute to colony composition throughout her lifetime. The potential colony genotype can therefore be conceptualised as the combination of the queen genome and all possible combinations between future recombinant oocytes and the genomes contributed by mating drones.
where:
- represents all possible maternal haplotypes generated through meiotic recombination,
- represents the set of haploid genomes contributed by mating drones,
- denotes all possible combinations between maternal and paternal haplotypes.
Under the assumptions of sperm viability, continued queen fertility, and complete sperm mixing, this potential genotypic space encompasses all worker genotypes that may be produced during the queen’s lifetime. This formulation can be expanded as:
where:
- is the recombinant oocyte genotype,
- is the haploid genome of the mating drone,
- is the total number of potential oocytes produced during the queen’s lifetime,
- is the number of effective mating drones.
One potentially informative approach would be to sequence both the queen and the sperm stored within her spermatheca. This could provide a direct estimate of the colony’s potential genotypic space by characterising both maternal and paternal genetic contributions available for future offspring production. However, because such an approach requires sacrificing the queen, its practical application remains limited.
However, only a fraction of this potential genotypic space is represented within the colony at any given moment. In theory, all patrilines generated from the stored sperm have the potential to contribute to colony composition. In practice, their relative representation may change through time. Workers from different patrilines can differ in behaviour, physiology, disease susceptibility, longevity, learning ability, and task allocation [71,72,74]. Consequently, environmental and social conditions may not affect all subfamilies equally. Disease outbreaks, parasite pressure, nutritional stress, climatic variation, demographic changes, or behavioural specialisation may alter the relative contribution of different patrilines to colony function.
As a result, the realised colony genotype may be viewed not simply as a random subset of the potential genotype, but as the outcome of continuous ecological and social filtering processes acting on genetically diverse subfamilies. Consequently, the relative contribution of different patrilines to colony function may vary through time despite a stable queen genotype and mating history. This distinction between potential and realised genotype is particularly relevant in eusocial organisms, where colony phenotype emerges from the collective activity of thousands of individuals whose relative genetic contributions may vary according to environmental and social context.
Recent genomic approaches such as pooled whole-genome sequencing (Pool-Seq) provide useful estimates of colony-level allele frequencies while reducing sequencing costs [80,81]. Nevertheless, such methods do not reconstruct individual patrilines, pedigree structure, or temporal changes in genotype representation. Sequencing a single worker captures only one recombinant genotype among thousands, whereas sequencing the queen reveals only the maternal component of colony diversity.
Despite major advances in genomics, comprehensive characterisation of the genetic architecture of an entire eusocial colony remains beyond current practice. Accurate description of colony genotype would require the genotyping of large numbers of individuals sampled repeatedly through time, allowing reconstruction of patriline diversity, demographic turnover, and temporal variation in genetic composition. These limitations have important implications for colony phenotyping, breeding value estimation, conservation genetics, and the development of biologically realistic breeding programmes.
This perspective naturally leads to a further question: if colony phenotype depends not only on the presence of multiple genotypes but also on their relative representation and interactions within the social environment, to what extent do genotype-by-genotype interactions contribute to colony-level traits?
2.5.5. Genotype-by-Genotype Interactions
In honeybee colonies, thousands of workers belonging to different patrilines cooperate, compete, and influence one another’s development and behaviour. Consequently, colony-level phenotypes cannot always be predicted from the additive effects of individual genotypes alone. Genetic subfamilies may differ in behavioural tendencies, task allocation, learning ability, disease resistance, physiology, longevity, and responsiveness to environmental stimuli [71,72,74]. Through social interactions, these differences can generate non-additive effects whereby the phenotypic contribution of a genotype depends partly on the genetic composition of the surrounding social environment.
At the colony level, phenotype emerges from continuous interactions among thousands of genetically heterogeneous individuals belonging to multiple patrilines and operating within a socially integrated superorganism. These interactions are mediated through pheromonal communication, trophallaxis, vibrational signalling, brood care, collective defence [82], thermoregulation, and foraging recruitment [83]. Queen mandibular pheromones regulate worker reproduction, behaviour, and gene expression [84,85], whereas brood pheromones influence nurse physiology and colony nutritional organisation [86,87]. Similarly, trophallaxis enables not only food exchange but also the transfer of hormones, proteins, microbiota, and signalling molecules among colony members. Through these behavioural and physiological feedbacks, genetically diverse workers become integrated into a coordinated social system whose collective properties cannot be inferred from isolated individuals alone.
Consequently, the honeybee colony can be viewed as a distributed biological information-processing system [73,88,89], in which thousands of interacting genomes collectively generate emergent phenotypes that cannot be predicted from isolated individuals alone.
Within this framework, colony phenotype emerges from both the genetic composition of the colony and the interactions occurring among its constituent genomes. Such interactions may influence gene expression, behaviour, physiology, and colony organisation, generating forms of social epistasis that extend beyond classical individual-based genetic models [82,88,90]. Colony performance therefore depends not only on the diversity of genotypes present, but also on how these genotypes interact and are organised within the social network of the superorganism.
A conceptual extension of the colony genotype framework that incorporates social genetic interactions may be expressed as:
where:
= genotype-dependent interactions between the queen and worker populations
= genotype-dependent interactions among workers
The colony genotype framework can therefore be conceptually extended to include not only the genetic composition of queens and workers, but also the interactions occurring among these genotypes. Colony phenotype emerges not only from the identities of the genotypes present, but also from the network of interactions linking them. Such interactions may occur between the queen and workers, among workers belonging to different patrilines, and among groups of individuals performing different social functions within the colony.
As Moritz et al. [91] anticipated, understanding honeybee genetics ultimately requires moving beyond the description of patriline frequencies toward the characterisation of interactions among genetic subfamilies. The ability to identify, isolate, phenotype, and quantify these interactions may prove essential for disentangling the complex genetic architecture underlying emergent colony-level traits.
The existence of genotype-by-genotype interactions further complicates the relationship between colony genotype and colony phenotype. Colony performance therefore emerges not only from the presence of genetic diversity, but also from the way that diversity is organised and expressed within the social environment of the colony.
Consequently, intracolonial genetic diversity should not be viewed solely as the coexistence of multiple genotypes, but also as a network of interactions among those genotypes. Understanding how these interactions contribute to emergent colony phenotypes remains a major challenge for honeybee genetics, breeding, and conservation.
Yet intracolonial genetic interactions represent only one component of a broader evolutionary system. The mechanisms by which colonies reproduce, exchange genetic material, and are exposed to natural selection further shape the distribution of genetic diversity within populations. These population-level processes are examined in the following sections.
At the colony level, phenotype emerges from continuous interactions among thousands of genetically heterogeneous individuals belonging to multiple patrilines and operating within a socially integrated superorganism (Figure 4).
These interactions are mediated through pheromonal communication, trophallaxis, vibrational signalling, brood care, collective defence [82], thermoregulation, and foraging recruitment [83]. Queen mandibular pheromones regulate worker reproduction, behaviour, and gene expression [84,85], whereas brood pheromones influence nurse physiology and colony nutritional organisation [86,87]. Similarly, trophallaxis enables not only food exchange but also the transfer of hormones, proteins, microbiota, and signalling molecules among colony members. Through these behavioural and physiological feedbacks, genetically diverse workers become integrated into a coordinated social system whose collective properties cannot be inferred from isolated individuals alone.
Consequently, the honeybee colony can be viewed as a distributed biological information-processing system [73,88,89], in which thousands of interacting genomes collectively generate emergent phenotypes. This perspective raises a fundamental question for honeybee genetics and breeding: if colony phenotype emerges from the interaction of thousands of recombinant genomes.
2.6. Colony Reproduction and Selection as Drivers of Mass Selection and Sustainable Breeding
Swarming is the primary natural mode of colony reproduction in A. mellifera, also called colony fission. The production of swarms is itself influenced by colony genotype, queen age, colony demography, and environmental conditions [22]. When colony population size, brood area, pheromonal signalling, or nest congestion exceed regulatory thresholds the colony initiates swarm preparations [23].
The mother colony produces multiple queen cells, and approximately one-third to one-half of the workers—along with the old queen—leave to establish a new nest site. This process results in the spatial redistribution of colonies across the landscape and creates opportunities for colonizing new or marginal environments.
Swarming has major evolutionary implications. Because the departing swarm carries a subset of the original colony’s genetic diversity—largely defined by the queen’s mate number and patriline composition—the founding colony represents a genetic “sample” of the parental superorganism. At the same time, the parent colony rears a replacement queen that will subsequently undertake mating flights and acquire a new combination of drone genotypes [22,23]. In some highly swarm-prone colonies, additional virgin queens may also depart in secondary or tertiary swarms, a tendency that varies among subspecies and breeding lines [92]. Consequently, colony reproduction through swarming generates new colonies that differ genetically from one another despite sharing a common origin. Through this process, genetic diversity generated by recombination and polyandry is continuously redistributed among colonies and across the landscape.
Following establishment, newly founded colonies face a series of ecological challenges, including nest-site suitability, resource availability, climatic constraints, pathogen pressure, and overwinter survival. Colony mortality can be substantial, with overwinter losses often ranging between 10 and 30% depending on environmental conditions [93]. As a result, swarming acts as the reproductive engine of honeybee populations, whereas natural selection acts as a filtering process that eliminates poorly adapted colonies while favouring those best suited to local conditions. Colonies that survive these environmental filters subsequently contribute disproportionately to the next generation through swarming and drone production, thereby increasing the representation of successful genetic combinations within local populations. In many respects, this process resembles a naturally operating population-level selection system, in which large numbers of newly founded colonies are continuously subjected to environmental evaluation and selective filtering. Unlike managed breeding programmes, however, selection is performed directly by local ecological conditions rather than predefined human criteria.
This combination of colony reproduction and selective filtering creates a self-organising evolutionary system operating at the population level. Recombination, polyandry, and independent mating events continuously generate novel genetic combinations; swarming redistributes this diversity among colonies and across landscapes; and natural selection filters these combinations according to local environmental conditions. Together, these processes generate a continuous cycle of diversity generation, redistribution, and filtering that promotes adaptation while maintaining evolutionary potential within honeybee populations.
2.7. From the Genetic Colony-Level to the Genetic Population-Level
At the population level, the genotype of each honeybee colony is not an isolated entity but a mosaic reflection of the surrounding regional gene pool. Through polyandrous mating at drone congregation areas, queens acquire genetic material from numerous drones originating from different colonies, thereby linking the genetic composition of individual colonies to broader population-level processes. Swarming further contributes to this connectivity by redistributing colonies and their genetic diversity across the landscape.
This organisation means that genetic variation is not confined within colonies but is continuously generated, exchanged, redistributed, and filtered across generations. Recombination and independent mating events generate new genetic combinations; polyandry and gene flow connect colonies within regional populations; swarming redistributes colony-level genetic diversity spatially; and natural selection filters this diversity under local environmental conditions. Thus, colony phenotypes emerge not only from the genetic composition of individual colonies, but also from the broader genetic and ecological context in which they are embedded.
The long-term consequences of these processes are illustrated by the emergence of distinct Apis mellifera subspecies and ecotypes, each characterised by specific combinations of behavioural, physiological, morphological, and life-history traits [24,92]. Over thousands of generations, local populations have been shaped by interactions among genetic diversity, environmental heterogeneity, and natural selection, producing adaptive phenotypic variation across contrasting ecological regions.
Consequently, honeybee colonies should not be considered only as units of production or management, but also as components of larger evolutionary systems. Understanding honeybee biology therefore requires extending the focus beyond individual colonies toward populations as the primary framework within which genetic diversity contributes to adaptation, resilience, and long-term evolutionary potential.
2.8. Adaptive Outcomes Through Honeybee Biology Natural Mechanisms
Honeybee-specific mechanisms of genetic diversification collectively increase genetic diversity within colonies and populations. Although these mechanisms differ in their biological nature, they converge toward a common outcome: the generation and maintenance of high levels of genetic variation. The recurring association between genetic diversity and colony-level performance across a wide range of biological functions suggests that genetic diversity is not merely a consequence of honeybee reproductive biology (Box 2). Rather, it appears to be an integral component of colony organisation and functioning, influencing multiple aspects of reproduction, behaviour, physiology, health, and fitness.
| Box 2. Effects of intracolonial genetic diversity on honeybee colony performance. |
Genetic diversity:
|
3. Non-Genetic Effects on Phenotypic Variation and Genotype by Environment Interactions
Phenotypic variation among honeybee colonies arises not only from genetic architecture and reproductive processes, but also from a wide range of environmental, ecological and management-related factors. These non-genetic drivers can act synergistically or antagonistically, may vary at multiple spatial and temporal scales, and often interact with colony demography and genotype, making their independent assessment particularly challenging. Because these influences cannot be experimentally controlled or replicated in identical conditions across years, establishing causal relationships between specific environmental variables and colony-level traits remains difficult.
Non-genetic determinants operate at two hierarchical levels:
Colony-site level, including microenvironmental conditions such as hive orientation, shade, wind exposure, nest substrate, temperature buffering capacity, and local floral resource patches. These variables are difficult to isolate experimentally as exact site conditions are unique to each colony.
Apiary-site level, encompassing landscape composition, climate, forage diversity and continuity, disease pressure, pesticide exposure, and beekeeper management. Although these conditions are more amenable to comparative or long-term studies, such work requires substantial monitoring effort and extensive environmental measurements, including: light intensity, temperature fluctuations, water availability (rainfall, hygrometry, dew), plant species richness and floral abundance, pollen availability and seasonal pollen flows, nectar flow dynamics, soil type and associated vegetation structure, ecosystem composition and succession, circadian rhythm perturbations, seasonality, climate change impacts, environmental toxicants, pathogen and parasite prevalence, beekeeping practices such as colony density, queen replacement, colony splitting, supplemental or artificial nutrition., varroa management, treatments, honey/pollen harvesting, shifting.
The central challenge is determining how to isolate the effect of a single non-genetic factor, given that environmental and management-related drivers typically covary. Additionally, the repeatability of experiments across years and regions is limited. Consequently, significant phenotypic variation is expected both among and across apiaries exposed to distinct environmental landscapes and management regimes.
3.1. Beekeeping Practices and Their Influence on Colony Phenotype
Large-scale surveys demonstrate that beekeeping practices can override or reinforce environmental stressors [125]. In addition, genetic-by-management interactions influence colony productivity and survival, with certain genotypes performing better under specific beekeeping conditions [126], i.e., colonies re-queening [127], migratory beekeeping can increase exposure to pesticides but improve forage access [128], colony density affects disease transmission dynamics [129], feeding practices modulate brood area and foraging recruitment [130,131] and disease-control treatments influence parasite loads, pathogen prevalence, colony survival, and productivity [132,133,134]. Thus, management decisions can amplify, buffer, or transform phenotypic expression.
3.2. Environmental and Nutritional Determinants of Honeybee Phenotype
Environmental conditions and nutritional resources shape honeybee phenotypes across three interconnected biological scales: the individual bee, the colony, and the population of colonies. Because honeybees rely exclusively on floral resources for their nutritional needs, the composition and diversity of the surrounding landscape directly influence the physiological, behavioural, and developmental traits of both workers and queens [135,136]. These individual-level traits, in turn, scale up to affect colony-level performance, resilience, and fitness. Furthermore, apiary density may modulates resource availability. Remarkably, although numerous studies have investigated potential competition between managed honey bees and wild pollinators [137,138], the extent to which managed honey bee colonies compete with one another for floral resources remains poorly documented. Even less is known about potential intraspecific competition between managed colonies and wild endemic honeybee populations occupying the same landscape. Nevertheless, increasing colony densities are expected to increase local demand for nectar and pollen resources, particularly when floral resources are limited.
3.2.1. Individual-Level Phenotype: Physiological, Developmental, and Behavioural Responses
Environmental and nutritional conditions exert profound effects on the phenotype of individual honeybees, from oocyte provisioning in queens, eggs, larva, pupa through to adult life. These effects are mediated by both the genetic background of the queen and workers, and the colony’s nutritional status [139,140,141]. Queens adjust egg size and provisioning in response to colony size and food availability [140,142], with smaller colonies receiving larger eggs and starvation leading to increased egg investment. Egg weight and viability are modulated by queen age, season, brood nest temperature, and genetic stock [64,143,144,145,146]. Additionally, workers can influence egg-laying rate and potentially egg characteristics [141].
At the molecular level, maternally-derived RNAs and proteins stored in oocytes influence early embryonic fitness and may shape later phenotypes [147,148,149]. Vitellogenin (Vg), whose synthesis is influenced by colony nutrition, also mediates trans-generational immune priming by binding pathogen fragments (PAMPs), thereby enhancing embryo resistance before hatching [150,151,152]. The mTORC1 pathway has been proposed to regulate oocyte provisioning under nutritional stress [153].
During larval development, the rate of growth, weight gain, and organ differentiation are highly sensitive to nutrition and environmental cues [145,154,155]. Larvae can increase their body mass ~1500-fold before pupation, fueled by protein- and lipid-rich diets, notably royal jelly [145]. Larval fat body development, critical for endocrine signaling and metamorphosis, follows a tightly regulated trajectory modulated by nutrient availability [156,157,158,159]. Environmental parameters including colony strength, brood temperature, humidity, pollen availability, and disease presence significantly affect larval physiology [145,160,161].
Nutrition is a key mechanistic driver of these developmental differences. In A. mellifera, caste determination provides the most striking example: variation in larval diet composition is sufficient to direct genetically identical larvae toward queen or worker developmental trajectories [162,163,164].
In adult workers, the quality and diversity of pollen diets influence immune gene expression [165,166], hypopharyngeal gland development [167,168], vitellogenin levels [169], and detoxification capacity [170]. Disease tolerance [171,172], lifespan [173,174,175,176], and behavioral maturation also respond to nutritional quality. Environmental variation modulates these nutritional pathways. Workers from florally diverse landscapes exhibit improved immunity, gland development, and longevity, while those from impoverished habitats show reduced physiological function [173]. Poor or imbalanced nutrition thus constrains individual phenotypic potential and narrows the colony’s pool of functional traits.
3.2.2. Colony-Level Phenotype: Emergent Properties and Superorganism Performance
Colony phenotype emerges from the aggregate physiological states, behavioural interactions, and task allocations of thousands of workers—each shaped by their nutritional and environmental experiences. Consequently, landscape-driven variation in forage quality and quantity translates into measurable colony-level outcomes.
Environmental heterogeneity and floral resource availability influence brood viability and brood area [177,178], colony growth rate [179,180], seasonal population dynamics [173,181,182], pathogen prevalence, including viral loads and Varroa-associated stress [183,184,185,186], foraging behaviour and efficiency, including recruitment, learning, and landscape exploitation [187,188,189], overwinter survival, a major determinant of colony fitness [93,184,190,191].
Colonies situated in simplified agricultural landscapes often experience nutritional bottlenecks resulting in reduced brood rearing [192,193], destabilised microbiome composition [194], impaired thermoregulation [195,196], heightened disease susceptibility, and lower overwinter survival. Although supplemental feeding can mitigate acute shortages, artificial diets do not fully reproduce the biochemical complexity or functional benefits of natural pollen.
The strong dependence of both individual and colony-level traits on the proximate nutritional environment highlights the complexity of phenotyping in honeybees. In this context, nutrigenomics and nutrigenetics provide complementary frameworks to disentangle GEI, by investigating how genetic variation modulates nutritional responses and how diet influences gene expression profiles, respectively. These approaches offer valuable insights into the mechanisms driving phenotypic plasticity and colony performance under variable environmental conditions.
3.2.3. Nutrigenomics: Gene Expression Responses to Nutrition
Nutrigenomics study how dietary inputs regulate gene expression, physiological states, and functional outcomes at the molecular level. In honeybees, this field offers a mechanistic framework to understand how nutrition influences developmental and behavioural plasticity, disease resistance, and social organisation. Because bees rely entirely on floral resources for essential nutrients even subtle differences in dietary composition can elicit substantial changes in gene expression.
Recent findings align with earlier theories of nutritional-social interactions in eusocial insects, where variation in individual nourishment and endocrine responses governs caste differentiation and division of labour [197]. Nutrigenomic studies have since shown that dietary variation modulates multiple molecular systems in honeybees:
Immune function: Protein-rich, diverse pollen diets upregulate key immune genes (e.g., defensin, hymenoptaecin, abaecin), enhancing pathogen resistance and colony resilience [165]. Conversely, poor nutrition suppresses immune expression and increases disease susceptibility [165,169].
Detoxification and oxidative stress: Nutritional enrichment boosts expression of detoxification enzymes (e.g., P450 monooxygenases, glutathione S-transferases) and antioxidant pathways, improving bees’ capacity to manage pesticides and environmental toxins [166].
Physiological development: Nutrient-driven expression profiles modulate glandular activity (e.g., hypopharyngeal glands), tissue differentiation, and caste development trajectories [166,174].
Endocrine activity and behavioural maturation: Diet affects juvenile hormone and vitellogenin levels, regulating the timing of task transitions (e.g., from nursing to foraging). Nutritional deficits accelerate these transitions, often reflecting colony stress [198].
Gut microbiome: Diet modulates gut microbial composition, and microbial metabolites influence neurophysiological gene expression [199,200] and behavioural responsiveness [201]. This diet–microbiome–brain axis introduces an emerging dimension of nutrigenomics
Together, these studies establish nutrition as a central molecular integrator linking environment to gene regulation, immune competence, detoxification capacity, endocrine signalling, and cognitive performance—thereby shaping colony-level phenotype and resilience.
3.2.4. Nutrigenetics: Genotype by Nutrition Interactions
Nutrigenetics explores how genetic variation modulates an organism’s response to nutritional environments. In the honeybee superorganism, this interaction is especially complex due to intracolonial genetic diversity arising from polyandry. Each colony comprises multiple worker subfamilies (patrilines) sharing the queen’s highly recombined genome but differing in their paternal haplotypes. This genetic mosaic produces divergent physiological and behavioural responses to the same nutritional inputs.
At the worker subfamily level, studies have demonstrated consistent patriline-specific variation in traits directly or indirectly linked to nutrition: Gustatory responsiveness and sugar sensitivity influence food acceptance and foraging recruitment [202,203], task thresholds and activation levels vary with genotype, modulating labour division [69,204,205], foraging specialisation (nectar vs. pollen) and starvation resistance show genetic determinism [21,206], Developmental and behavioural maturation vary by genotype [207], as does microbiome composition, which affects nutrient assimilation and neural functioning [208,209].
At the colony level, genetic diversity generated by queen polyandry translates into enhanced nutritional resilience and performance. Colonies with higher patriline diversity exhibit improved brood rearing, pollen collection, food conversion, and overall productivity, particularly under variable or limited resource conditions [109,124]. This diversity increases the likelihood that some subfamilies possess genotypes better suited to specific nutritional environments, promoting functional complementarity. Such intracolonial variation ensures a broader range of gustatory sensitivity, metabolic capacities, and behavioural plasticity among workers [101,110,118,210] thereby buffering colonies against nutritional stress and supporting stable development and immune function in heterogeneous landscapes.
At the subspecies level, geographic races of A. mellifera (e.g., A. m. mellifera, A. m. ligustica or A. m. carnica) exhibit genetically shaped nutritional ecotypes adapted to local floral landscapes, climatic conditions, and disease pressures [211,212,213].
Altogether, genotype by environment interactions (GEI) are major drivers of honeybee phenotypic plasticity, colony performance, and local adaptation. Recognising these interactions is essential for developing population-based breeding strategies integrated with landscape-scale conservation programmes, as colony fitness ultimately emerges from the interplay between intracolonial genetic diversity and environmental heterogeneity. However, these interactions are not static. Their magnitude and direction may vary throughout development, across worker age classes, between seasons, and among years. Consequently, understanding honeybee phenotypes requires considering time as a third fundamental dimension interacting with both genotype and environment, leading to a G×E×T framework.
4. Temporal Dynamics in Honeybee Phenotypes: G×E×T Framework
Time is a central dimension shaping honeybee phenotype at multiple scales. Because colony-level traits result from the dynamic interplay between genotype, environment, and within-colony demography; temporal fluctuations—both across years and within a single season—profoundly influence the expression of behavioural, physiological, and productivity-related traits. These shifts create challenges for phenotypic assessment, experimental repeatability, and interpretation of trait variation within and between colonies.
Importantly, environmental conditions themselves are not static but fluctuate continuously through time. Floral resource availability, climatic conditions, pathogen pressure, pesticide exposure, and colony density all vary across daily, seasonal, and interannual timescales. Consequently, colonies experience Environmental by Time interactions, whereby the nature and intensity of environmental pressures change over time. These fluctuations generate shifting selective landscapes that continuously modify colony performance, survival, and reproductive success. Under such conditions, adaptation depends not only on the ability of colonies to respond to a given environment, but also on their capacity to cope with environmental variability itself.
4.1. Across-Year Dynamics: Short Colony Lifespan and r-Strategy
Compared with classical livestock species, the honeybee colony—considered as a superorganism—has a short functional lifespan. While rare colonies may persist for 5–8 years [93,214], typical unmanaged colonies rarely survive beyond three years [215], and modern apiculture practices, including annual requeening and treatment-related stress, often reduce this to a single season of effective productivity [216].
Honeybee colonies follow an r-selected reproductive strategy, characterised by rapid population expansion, early reproduction, and the frequent generation of new colonies via swarming. Empirical estimates indicate that while only ~10% of first-year colonies initiate swarming, this probability increases to ~30% in the second year and ~50% by the third [217]. Consequently, colony identity is not temporally stable: it shifts through processes such as natural swarming, supersedure, and queen turnover, often leading to changes in both genotype (via queen replacement) and phenotype (via altered demography and environment interaction).
These demographic events introduce temporal drift in observed traits, making it difficult to attribute phenotypic differences across years to genetic factors alone. Observed trait variation may be confounded by environmental noise, colony ageing, pathogen load accumulation. Therefore, multi-year comparisons between colonies must be interpreted cautiously, as they rarely reflect genotype in isolation, but rather composite outcomes of genotype, environment, and time.
Figure 5.
Theoretical honeybee colony demography overtime in temperate climate with spring and autumn colony development.
Figure 5.
Theoretical honeybee colony demography overtime in temperate climate with spring and autumn colony development.
4.2. Within-Season Dynamics: Resource and Demography
Seasonal variation adds a second layer of complexity to phenotypic expression. The timing, quantity, and quality of the spring pollen flow is a major determinant of early colony growth, with nutrient-rich pollen stimulating brood production [218], hypopharyngeal gland development [219], and forager recruitment [220]. Conversely, summer dearths, late-season blooms, or climatic anomalies (e.g., heatwaves, drought) can constrain floral resource availability, leading to nutritional stress and shifts in colony dynamics. Reduced pollen intake alters brood quantity and quality [220], impacts worker lifespan and turnover rates [221], and decreases the expression of resistance traits against parasites and pathogens [171,222]. Foraging intensity and pollen source preference are modulated in response to changing resource landscapes [218,223], often favouring low-quality or previously avoided plants [224]. These behavioural shifts are accompanied by changes in hygienic behaviour and grooming responses [225], potentially weakening colony defence mechanisms. As a result, colony-level productivity, queen replacement dynamics, and swarming probability may be altered [226]. Environmental unpredictability further accentuates inter-colony variation in growth and performance, even under similar genetic backgrounds [227]. Such seasonal fluctuations highlight the need to assess colony phenotypes within a temporal and ecological context.
Further, honeybee colonies undergo rapid demographic renewal during the active season. Summer workers live only 30 to 50 days, meaning the entire colony workforce turns over several times during a season. Each new age-cohort composed by several genetics subfamilies reflects a different age structure, metabolic state, immune readiness, and behavioural role. This internal demographic flux is not neutral: because many colony-level traits (e.g., foraging intensity, hygienic behaviour, thermoregulation) are age-structured and depend on subfamilies genotype, phenotypic outputs will vary significantly depending on when a colony is sampled.
In contrast, winter bees, physiologically distinct with higher vitellogenin levels and lipid reserves, live 120–180 days and bridge the seasonal foraging gap. The transition between summer and winter phenotypes involves complex hormonal and behavioural shifts, which are in turn shaped by colony nutritional status, photoperiod, temperature, and pathogen pressure [228]. Thus, colony phenotype across a season is never static, but rather moves through a succession of transient equilibria, each shaped by internal demography and external ecological conditions.
Consequently, colony phenotype should be understood as an environment-dependent and time-sensitive emergent property rather than a fixed attribute of a stable biological individual. Environmental conditions continuously fluctuate through time, modifying the selective pressures experienced by colonies and generating strong Environment by Time interactions. Simultaneously, colony demography undergoes continuous renewal, with changing age structures and differential contributions of worker subfamilies to colony activities. Consequently, the effective genotype expressed at the colony level may itself vary through time as different patrilines contribute disproportionately to behavioural, physiological, and social functions [229]. Colony phenotype therefore emerges from the dynamic interaction between genotype, environment, and time, highlighting the necessity of adopting a G×E×T framework when studying honeybee biology, phenotyping, breeding, and conservation.
5. Phenotyping Through GxExT
The preceding sections demonstrate that honeybee phenotypes emerge from the interaction of complex genetic architectures, heterogeneous environmental conditions, and temporal dynamics operating simultaneously at multiple biological scales. Unlike most domesticated livestock species, where individuals can be phenotyped and selected as relatively stable biological entities, honeybee colonies are transient superorganisms characterised by continuous demographic turnover, potential shift among patriline frequencies, age-dependent task allocation, fluctuating environmental conditions, and dynamic social interactions.
Consequently, phenotypic measurements obtained from a colony represent only a temporal snapshot of an underlying biological system that is constantly changing. Colony phenotype is therefore not a fixed property but a dynamic expression of G×E×T interactions. These characteristics create major challenges for phenotyping design, trait interpretation, genetic evaluation, and breeding strategies.
5.1. Emergent Phenotype of Honeybee Colony: The Functional Unit of Selection
In A. mellifera, colony phenotype arises from the integration of multiple biological hierarchies—individual bees, age cohorts, genetic subfamilies, and their interactions with environmental variables across time. This emergent phenotype reflects the superorganism nature of the colony and is considered the primary unit of selection in both ecological and breeding contexts.
The performance of a colony is not a simple additive function of individual traits, but an emergent property that emerges from interactions among colony components and whose expression varies through time. As such, colony traits are inherently interdependent [230]. For example, high honey production alone does not define a high-quality colony if it is accompanied by poor disease resistance, low overwintering survival, or excessive swarming tendency. Colony-level traits are typically polygenic and quantitative, resulting from the interaction of multiple genetic loci combined with environmental and management influences. Moreover, these traits are strongly contextual and plastic, being modulated by colony age, seasonal dynamics, local environmental conditions, resource availability, and beekeeping practices. Consequently, colony phenotype should be interpreted as a dynamic, integrative expression of genetic potential shaped continuously by environmental and temporal factors.
The dynamic interplay of G×E×T interactions complicate the assessment of colony performance over short timescales and calls into question the relevance of phenotyping at isolated biological levels. While individual-level measurements (e.g., worker physiology, foraging behaviour, queen reproductive traits) provide mechanistic insights, they fail to capture the integrated, emergent properties of the colony. Similarly, caste-specific, age-group-specific, or patriline-level traits are informative but insufficient in isolation. Nevertheless, phenotyping at these lower biological levels remains essential for understanding the mechanisms underlying colony function. Measurements performed on individual queens, workers, drones, brood stages, age cohorts, or genetic subfamilies have provided major insights into behavioural maturation [72,83], division of labour [21,71], reproductive biology [17,22], nutritional physiology [165,166,183], disease resistance [20,231,232], social immunity [82], and the consequences of polyandry [90,115,124]. Likewise, some measurements performed on only a few individuals—or even a single bee—such as mitochondrial haplotypes, wing morphometrics, genomic markers, or pathogen screening, can provide valuable information on lineage identity, introgression, population structure, genetic diversity, disease status or colony health. Such approaches are therefore indispensable for mechanistic, genetic, and conservation studies. However, they describe specific biological components rather than the integrated expression of colony performance.
Given that colony function arises from the interaction among these subunits, the emergent colony phenotype represents the lowest biologically meaningful level of phenotypic assessment. It is at this level that biological processes such as brood production, disease resistance, foraging dynamics, and productivity manifest holistically.
A finer decomposition of worker–worker interactions () may be expressed as:
This formulation integrates both genetic stratification (via patriline identity) and temporal/demographic dynamics (via age cohorts), acknowledging that worker behaviour, physiology, and influence on colony performance vary across both lineage and life stage. Such an approach opens the door to social epistasis analysis, where subfamily identity and temporal structure become central variables in breeding and experimental design.
Therefore, if we consider the phenotype of a colony () as an emergent property resulting from genetic, social, and environmental interactions at a specific time (t), a conceptual expression can be proposed:
where:
- = the phenotypic contribution of the queen (e.g., egg-laying rate, pheromone production, genotype)
- = the aggregated phenotypic effects of the worker population (from multiple patrilines and age classes)
- = Interactions between the queen and her worker offspring
- = Social genetic and age group interactions among workers
- = environmental effects (nutrition, climate, landscape, pathogens, management)
- = genotype-by-environment interactions, which modulate trait expression under different ecological or management contexts
This formulation underscores the multi-level and dynamic nature of colony phenotypes, where individual contributions are embedded within a network of social and ecological interactions. Importantly, these interaction terms are non-additive and often non-linear, meaning that emergent colony traits (e.g., hygienic behaviour, thermoregulation, productivity) cannot be inferred simply by summing individual phenotypes. Moreover, the relative contributions of each term may vary over time, as worker cohorts are replaced, potential sperm use shifts, and environmental conditions fluctuate. This highlights the temporal dimension of colony phenotype architecture, further justifying the inclusion of time in the theoretical frameworks as G×E×T interactions.
5.2. Limitations of Current Phenotyping Approaches
Despite considerable efforts to standardise honeybee breeding and performance evaluation, phenotyping remains one of the major limitations of selection programmes. Most colony traits are inherently complex because they emerge from the interactions among thousands of individuals, their environment, and temporal dynamics. As a result, obtaining phenotypic measurements that accurately reflect colony genetic potential remains challenging.
Many traits routinely assessed in breeding schemes rely on semi-quantitative scoring systems based on observer perception, including aggressiveness, calmness on combs, swarming tendency, or hygienic behaviour [233,234]. Although practical for large-scale evaluations, such measurements remain partially subjective and may vary among observers, regions, management systems, and cultural contexts. Even apparently simple measurements, such as estimating colony population size or brood abundance, may differ substantially among operators.
A second limitation arises from the temporal nature of colony phenotypes. Most assessments are performed at a single time point or during a restricted period of the season. However, colony phenotype is continuously modified by demographic turnover, fluctuations in resource availability, climatic conditions, pathogen pressure, colony developmental stage, and seasonal processes. Consequently, the same colony may express markedly different phenotypes depending on when measurements are performed.
Furthermore, phenotypic observations often represent indirect proxies of underlying biological processes. Colony productivity, brood development, overwintering success, or behavioural traits emerge from complex interactions among genetic, environmental, physiological, nutritional, and social factors. Single measurements therefore rarely capture the full biological complexity underlying colony performance.
Together, these limitations indicate that phenotypic measurements should not be interpreted as fixed descriptors of colony genetic value. Rather, they represent context-dependent observations influenced by the interaction of genotype, environment, and time. Recognising this limitation is essential for developing more robust phenotyping strategies capable of supporting both breeding and conservation objectives.
5.3. Trait Classification Frameworks and Standardisation Challenges
Colony phenotyping has long been the cornerstone of honeybee breeding programmes. Large-scale European initiatives such as SMARTBEES and operational genetic evaluation systems such as BeeBreed have greatly contributed to the standardisation of performance testing protocols and the implementation of BLUP-based breeding value estimation at the colony level [235,236,237]. These programmes represent major advances towards data-driven selection and more objective evaluation of colony performance.
Nevertheless, further progress depends on the development of phenotyping approaches that are both more quantitative and more biologically informative. Traditional colony assessments often rely on relatively coarse indicators, such as visual estimates of adult bee populations, brood abundance, food reserves, or behavioural scores. While operationally efficient, these measurements may lack precision and can be influenced by observer bias and environmental conditions.
Recent technological developments provide opportunities to improve phenotypic characterisation. These include standardised measurements of brood area [238,239], quantitative estimation of colony population size [239,240], image-based assessment of brood and food stores [238,241,242] automated monitoring systems [243], behavioural tracking [244], and molecular or physiological indicators of colony condition. In addition, integrating information on the quantity, quality, and diversity of nutritional resources may provide a more comprehensive understanding of colony functional status and adaptive capacity [193,245].
However, implementing such approaches presents substantial practical challenges. Quantitative phenotyping is often labour-intensive, requires specialised equipment and trained personnel, and may require repeated measurements over multiple seasons or years to adequately capture temporal variability and G×E×T interactions. These constraints impose considerable logistical and financial burdens that currently limit their large-scale implementation.
Consequently, the challenge is not merely to increase measurement precision, but to develop phenotyping frameworks capable of capturing the dynamic and multilevel nature of honeybee phenotypes.
This perspective may require a shift in breeding philosophy.
Phenotyping should not be viewed exclusively as a tool for identifying a small number of elite colonies. Instead, it may serve to guide population-level adaptation by identifying colonies that consistently fail to meet predefined adaptive or production thresholds while maintaining broad genetic diversity among the remaining population. In such a framework, the objective shifts from maximizing the performance of a few exceptional colonies to progressively improving the adaptive performance of the breeding population as a whole. These considerations suggest that, although colonies remain the operational unit of phenotyping, the breeding population may represent the most appropriate biological unit for long-term genetic improvement. The implications of this shift in perspective are explored in the following section.
6. Population-Based Breeding and Conservation Frameworks
The previous sections have highlighted the remarkable complexity of honeybee phenotypes, which emerge from interactions among genetic variation, environmental heterogeneity, and temporal dynamics operating simultaneously at multiple biological scales. Unlike many livestock species, honeybee phenotypes are not solely determined by individual genotypes but arise from the collective functioning of colonies composed of thousands of interacting individuals, themselves embedded within larger populations connected through gene flow, mating systems, ecological interactions, and evolutionary processes [34,246,247,248,249].
These biological characteristics present both opportunities and challenges for selective breeding. Significant genetic progress has been achieved for traits such as honey production, hygienic behaviour, gentleness, spring development, and resistance to parasites through controlled mating and quantitative genetic approaches [250,251,252]. However, simulation studies and empirical breeding programmes have also revealed the potential consequences of intensive directional selection, including increased inbreeding, loss of genetic diversity, reduced effective population size, and erosion of adaptive potential [248,253,254].
In the context of rapidly changing environmental conditions, the challenge therefore extends beyond the identification of superior colonies. Climate change, emerging pathogens, novel pesticides, changing floral resources, and evolving management practices continuously modify the selective pressures experienced by honeybee populations.
Because energetic and nutritional resources are finite, colonies cannot maximise all biological functions simultaneously. Nutrients collected from the environment must be continuously allocated among brood production, maintenance, immunity, thermoregulation, detoxification, reproduction, and survival. Consequently, colony phenotypes emerge not only from genetic and environmental variation but also from resource allocation decisions that generate physiological and behavioural trade-offs. Understanding these trade-offs is therefore essential for interpreting colony performance and predicting responses to environmental change and selective breeding.
Consequently, breeding strategies optimized for present conditions may not necessarily maximize future adaptation. This raises a fundamental question: should honeybee improvement focus solely on maximizing current performance, or should it also aim to preserve the evolutionary processes that enable future adaptation?
The following sections examine this question by exploring the strengths and limitations of contemporary breeding approaches and by proposing a population-based framework in which breeding and conservation are viewed as complementary components of a broader adaptive management strategy.
6.1. From Colony Improvement to Adaptive Population Management
Traditional breeding programmes are largely based on the identification and propagation of superior individuals. This paradigm has been highly successful in many domesticated livestock species, where breeding objectives are generally focused on maximizing the frequency of desirable alleles associated with production, health, or behavioural traits. Similar approaches have been progressively implemented in honeybees through controlled mating stations, instrumental insemination, pedigree reconstruction, breeding value estimation, and BLUP-based selection schemes [250,251,252].
These methods have demonstrated that substantial genetic gains can be achieved for numerous colony-level traits of economic and biological importance, confirming that selective breeding remains an effective tool despite the biological complexity of honeybee colonies. Simulation studies consistently predict substantial genetic gains for colony-level traits under selective breeding. Using models that account for haplodiploidy, polyandry, and the combined effects of queens and workers on colony performance, [254] demonstrated strong improvements in breeding values over multiple generations of selection. Similarly, [248] and [253] predicted significant responses to selection for quantitative traits, particularly under mass-selection strategies.
These theoretical predictions are supported by empirical breeding programmes. The European BeeBreed initiative and the Canadian programme described by [252] both reported sustained improvements in traits such as honey production, hygienic behaviour, spring development, gentleness, and swarming tendency. Collectively, these studies demonstrate that selective breeding is a powerful tool capable of improving colony performance.
However, the reproductive biology and population structure of honeybees fundamentally differ from those of most domesticated animals. Queens mate with numerous drones originating from large mating populations, generating extensive gene flow through DCAs [11,57]. Furthermore, swarming, drifting, robbing behaviour, colony reproduction, beekeeper-mediated colony movements, and pathogen transmission continuously connect colonies within larger ecological and genetic networks. As a consequence, colonies cannot be considered fully independent breeding units but rather represent transient expressions of a broader population gene pool. Beyond gene flow, colonies are also ecologically interconnected through competition for floral resources, robbing behaviour, drifting workers, and pathogen transmission. Colony performance therefore depends not only on its own genetic composition but also on the ecological and epidemiological context generated by neighbouring colonies [129,255]. Such interactions reinforce the view that colony phenotypes emerge within population-level networks rather than as isolated expressions of individual genotypes.
This improvement is not achieved without evolutionary consequences. By definition, selection modifies allele frequencies, alters genetic variance, and changes population structure. Simulation studies consistently identify a trade-off between genetic gain and the maintenance of diversity. Mass selection generally produces greater genetic progress but also accelerates inbreeding and reduces effective population size [248,253]. In honeybees, these effects are particularly important because reduced allelic diversity at the csd locus increases the frequency of diploid drones and decreases brood viability. More recent simulations incorporating polyandry and colony-level genetic architecture reached similar conclusions, showing that mass selection generated higher performance gains but also substantially higher inbreeding levels, whereas polyandry reduced inbreeding while maintaining comparable genetic progress [254]. Thus, while selective breeding can effectively improve targeted traits, it simultaneously modifies the evolutionary properties of populations. From an evolutionary perspective, genetic diversity should not be viewed merely as a reservoir of neutral variation but as the substrate upon which future adaptation depends. Maintaining diversity is therefore not opposed to genetic improvement; rather, it is a prerequisite for the long-term sustainability of selection itself.
The challenge becomes even more pronounced when considering the dynamic nature of adaptation. The previous sections have shown that colony performance is not a fixed attribute but an emergent outcome of G×E×T interactions. Under such conditions, the phenotypes that maximize productivity under current environmental conditions may not necessarily confer optimal performance under future climates, novel pathogen pressures, or changing nutritional landscapes. Indeed, adaptation depends not only on the presence of favourable alleles but also on the capacity of populations to generate new phenotypic combinations through recombination, genetic diversity, and natural selection.
Consequently, the long-term objective of honeybee improvement may extend beyond maximizing colony performance alone and include the maintenance of adaptive evolutionary processes. This broader perspective shares important conceptual similarities with Darwinian beekeeping, an approach that advocates allowing natural selection to contribute to colony adaptation while reducing excessive reliance on human-directed selection [256,257,258,259]. Rather than focusing exclusively on the multiplication of a limited number of elite colonies, Darwinian approaches emphasize the adaptive value of population-level evolutionary processes, local adaptation, and natural selection acting under real environmental conditions [260].
While colony-level selection remains an essential component of breeding programmes, sustainable improvement may require maintaining the adaptive capacity of populations as a whole. From this perspective, honeybee breeding can be viewed not simply as the propagation of elite colonies but as a form of adaptive population management in which productivity, resilience, evolutionary potential, and conservation become interconnected objectives.
6.2. Selection Reshapes Evolutionary Trajectories Through Trait Interdependence and Trade-Offs
The consequences of selective breeding extend beyond changes in genetic diversity and inbreeding levels. By altering the frequency of specific alleles and trait combinations, selection influences the direction of evolutionary change itself. Consequently, breeding should not be viewed solely as a process of improving desirable characteristics, but also as a process that constrains alternative evolutionary trajectories.
This distinction is particularly important because colony performance emerges from numerous interconnected physiological, behavioural, developmental, and ecological traits. As a result, selection rarely acts on a single trait in isolation. Improvements in one component of colony performance may be accompanied by correlated responses in other traits due to pleiotropy, genetic linkage, physiological constraints, or resource allocation trade-offs. Such relationships are common throughout biology and reflect the finite energetic and developmental resources available to organisms [1,261,262,263].
Honeybee breeding provides several examples of this complexity. Selection for hygienic behaviour has successfully improved the removal of diseased or parasitized brood and contributed to enhanced colony health in many breeding programmes [251,252]. However, hygienic behaviour requires worker time, sensory activity, and colony resources that could otherwise be allocated to foraging, brood care, or other tasks. Although the net benefits of hygienic behaviour often outweigh these costs under current disease pressures, the existence and magnitude of associated trade-offs remain incompletely understood.
Although empirical evidence remains limited, physiological trade-offs may also occur at deeper biological levels. Colony productivity depends on the allocation of nutrients toward brood production, foraging activity, metabolic maintenance, immune function, detoxification processes, and long-term survival. For example, the insect fat body plays central roles in nutrient storage, immunity, oxidative stress responses, detoxification, endocrine regulation, and longevity [264,265]. Selection favouring rapid spring development, intense brood production, or high productivity may therefore influence physiological allocation patterns in ways that are not immediately visible through standard breeding evaluations. Although such mechanisms remain poorly explored in honeybee breeding, they illustrate how selection may favour particular adaptive strategies while reducing investment in alternative functions that become important under different environmental conditions.
The implications of these trade-offs extend beyond the traits directly targeted by breeders. Because selection acts on interconnected physiological, behavioural, developmental, and reproductive systems, it inevitably alters the range of phenotypic combinations available within populations. Consequently, breeding does not simply increase the frequency of desirable traits; it also determines which genetic combinations, adaptive strategies, and evolutionary pathways remain available to future generations. Selection therefore acts not only on present performance but also on the future evolutionary trajectory of honeybee populations.
6.3. Adaptive Potential as a Breeding Objective
6.3.1. Beyond Current Performance
Conventional breeding programmes are generally evaluated according to their capacity to improve colony performance over successive generations. Under relatively stable environmental conditions, such an objective is both logical and effective, as the traits contributing to productivity, health, and management suitability can be progressively enhanced through selection. The preceding section suggests that selective breeding influences not only current performance but also the evolutionary options available to future populations. This raises a further question: what should breeding programmes ultimately optimize?
A central assumption underlying most breeding programmes is that the phenotypes considered desirable today will remain advantageous in the future. Yet environmental conditions experienced by honeybees are becoming increasingly dynamic. Climate change is altering temperature regimes, flowering phenology, and resource availability. Pathogen communities continue to evolve, novel parasites and diseases emerge, pesticide exposure changes through time, and landscapes are continuously modified by agricultural intensification and urbanization. Under such conditions, future selective pressures cannot be predicted with certainty.
This uncertainty raises a fundamental question: what constitutes the value of a population? Traditional breeding frameworks often define population value according to the average performance of its colonies. However, evolutionary theory suggests that population value may also reside in its capacity to respond to future selective pressures. In other words, adaptation depends not only on the quality of existing phenotypes but also on the ability of populations to generate new phenotypic combinations when environmental conditions change.
From this perspective, adaptive potential may represent a distinct biological property that complements current performance. While colony productivity measures how well populations perform under present conditions, adaptive potential reflects their capacity to continue adapting under future conditions. These two objectives are not necessarily identical. A highly optimized population may achieve exceptional performance in a specific environment while simultaneously exhibiting reduced evolutionary flexibility if genetic diversity and alternative adaptive strategies have been eroded through prolonged directional selection.
Consequently, long-term sustainability may require balancing immediate genetic gain against the preservation of adaptive capacity. Such a balance does not imply abandoning selective breeding. Rather, it suggests that breeding programmes should consider not only which phenotypes are currently desirable but also how selection influences the evolutionary opportunities available to future generations.
6.3.2. Sources of Adaptive Potential
Adaptive potential emerges from multiple biological processes operating simultaneously within populations. Genetic diversity provides the raw material upon which natural and artificial selection can act. Recombination continuously generates novel combinations of alleles, while mutation introduces additional variation over longer evolutionary timescales. In honeybees, polyandry further contributes to intracolonial and population-level diversity by increasing the number of patrilines represented within colonies [98,266].
However, adaptive potential cannot be reduced to genetic diversity alone. The maintenance of locally adapted populations, ecological heterogeneity, behavioural variation, and phenotypic plasticity also contributes to the ability of populations to respond to changing environments.
Adaptive potential is also embodied in the locally adapted populations that have emerged throughout the natural range of A. mellifera. Numerous subspecies and regional ecotypes exhibit distinct combinations of morphological, behavioural, physiological, developmental, and life-history traits associated with local climatic conditions, resource availability, pathogen pressures, and seasonal constraints [24,211,212,267]. These populations can be viewed as evolutionary experiments conducted over thousands of generations, each representing a particular adaptive solution to a specific ecological context. Consequently, conserving locally adapted populations preserves not only genetic diversity but also adaptive strategies that may become increasingly valuable under future environmental change.
Throughout their evolutionary history, honeybee populations have adapted to highly diverse climatic conditions ranging from northern continental environments to Mediterranean, tropical, and arid regions. These adaptations emerged through long-term interactions among genetic variation, environmental conditions, and natural selection operating at population scales.
Importantly, adaptive potential is often difficult to measure directly because it concerns future possibilities rather than current performance. Colonies carrying rare alleles or uncommon trait combinations may contribute little to present breeding objectives while nevertheless providing critical evolutionary resources under future environmental conditions. Likewise, populations that appear suboptimal according to current production criteria may harbour adaptations that become advantageous under novel climatic, nutritional, or disease pressures.
The preservation of adaptive potential therefore requires maintaining not only genetic diversity but also the evolutionary processes that continuously generate, test, and reshape biological variation. In this sense, adaptation should be viewed as an ongoing population-level process rather than a fixed endpoint that can be permanently achieved through selection.
6.3.3. Reframing Non-Selection as an Adaptive Management Strategy
Within modern breeding programmes, non-selection is often perceived as the absence of genetic improvement. Under this view, populations that are not subjected to artificial selection are considered genetically stagnant or unmanaged, while selection is regarded as the primary mechanism through which adaptation and progress occur. Although this interpretation is understandable from a production-oriented perspective, it does not fully reflect the evolutionary processes operating within honeybee populations.
From a biological perspective, non-selection does not imply the absence of selection. Honeybee populations that are not subjected to artificial breeding continue to experience powerful selective pressures arising from climate, resource availability, pathogens, parasites, predators, competition, and colony reproduction. Natural selection continuously filters phenotypes through differential survival and reproductive success, favouring trait combinations that increase fitness within local environmental conditions. Consequently, unmanaged populations remain evolutionarily dynamic even in the absence of deliberate human intervention.
Several naturally surviving populations illustrate this principle. Feral colonies in the Arnot Forest in the United States persisted for decades despite the presence of Varroa destructor, demonstrating that adaptation can emerge under sustained natural selection [268,269]. Similar observations have been reported from untreated survivor populations on the island of Gotland in Sweden [270,271,272], in France [273], in Norway [274], in South Africa [275], and in long-term survivor-selection programmes conducted under commercial beekeeping conditions [276]. Collectively, these studies demonstrate that honeybee populations can evolve mechanisms allowing long-term persistence in the presence of Varroa destructor without systematic chemical control.
These observations are consistent with the principles of Darwinian beekeeping, which advocate management practices that allow natural selection to contribute to colony adaptation while minimizing unnecessary human intervention [277]. Similarly, survival-based approaches such as the “Bond test” developed by Kefuss and colleagues demonstrate that artificial selection can be partially aligned with natural selection by preferentially propagating colonies capable of surviving local environmental and parasite pressures without intensive intervention [276,278]. Together, these examples illustrate that breeding and natural selection need not be viewed as opposing forces. Rather, they can operate synergistically, with natural selection continuously filtering adaptive variation while breeders influence the direction and intensity of that filtering process. Importantly, such populations are not improving toward predefined production goals but toward increased fitness under local environmental constraints.
Nevertheless, the interpretation of these survivor populations remains an active area of debate. Survival does not necessarily imply the evolution of parasite resistance. Different populations may survive through reduced mite reproduction, behavioural resistance, altered colony demography, increased swarming, viral tolerance, or even reduced parasite virulence [275,279,280]. Consequently, selecting solely for colony survival may favour either resistance or tolerance mechanisms, which may have different epidemiological consequences. Recent analyses have highlighted that tolerance-based survival could permit the maintenance of higher parasite burdens and potentially increase pathogen transmission within managed and wild bee communities [281]. Distinguishing resistance from tolerance therefore remains essential when interpreting the outcomes of natural-selection-based breeding programmes.
This distinction highlights a fundamental difference between artificial and natural selection. Artificial selection typically focuses on a limited number of measurable traits that are considered desirable under current management conditions. Natural selection, in contrast, acts simultaneously on the entire phenotype and integrates a much broader set of ecological, physiological, behavioural, developmental, and reproductive factors. As a result, natural selection may preserve trait combinations whose adaptive value is not immediately apparent from production-based evaluations.
The concept of non-selection therefore deserves reconsideration. Rather than representing the absence of improvement, non-selection may function as a strategy for preserving evolutionary processes. Populations subjected to little or no artificial selection can maintain genetic diversity, rare alleles, locally adapted gene complexes, and alternative adaptive strategies that might otherwise be lost through strong directional selection. These populations may serve as reservoirs of evolutionary potential, providing the raw material from which future adaptations can emerge.
This perspective becomes increasingly relevant under conditions of environmental uncertainty. Because future selective pressures cannot be predicted with confidence, it is impossible to determine which genetic combinations will prove most valuable in coming decades. Under such circumstances, preserving a diversity of evolutionary trajectories may be as important as maximizing current performance. Consequently, non-selection should not necessarily be viewed as an alternative to breeding, but rather as one component of a broader adaptive management framework in which different levels of artificial selection coexist with natural evolutionary processes.
Viewed in this way, breeding and non-selection are not opposing strategies. Instead, they represent complementary approaches operating along a continuum of selection intensity. While intensive breeding can accelerate the improvement of specific traits, populations maintained under reduced or absent artificial selection can preserve the adaptive diversity upon which future improvement ultimately depends.
6.4. Integrating Breeding and Conservation
Historically, breeding and conservation have often been approached as distinct, and sometimes conflicting, objectives. Breeding programmes generally seek to increase the frequency of desirable traits through directional selection, whereas conservation initiatives focus on preserving genetic diversity, maintaining local populations, and limiting genetic erosion. This apparent opposition has frequently generated tensions between production-oriented and conservation-oriented approaches to honeybee management.
However, the preceding discussion suggests that such a dichotomy may be overly simplistic. Selective breeding depends fundamentally on the availability of genetic variation, while genetic variation itself is maintained through evolutionary processes operating within populations over time. Consequently, conservation and breeding are not independent activities but rather interconnected components of the same adaptive system.
The history of animal breeding repeatedly illustrates this relationship. Genetic improvement relies on the existence of heritable variation upon which selection can act. Whenever diversity becomes excessively reduced, selection responses tend to decline because populations approach genetic uniformity. In contrast, populations maintaining high levels of genetic variation retain a greater capacity to respond to both artificial and natural selection. Thus, conservation does not merely preserve historical genetic resources; it also safeguards the evolutionary potential required for future improvement.
This relationship may be particularly important in honeybees. The reproductive biology of the species, characterized by polyandry, extensive gene flow, colony-level selection, and strong environmental interactions, naturally promotes the generation and maintenance of diversity at multiple biological scales. Moreover, the broad geographic distribution of A. mellifera has produced numerous locally adapted populations shaped by distinct climatic conditions, pathogen communities, floral resources, and management histories [24,267].
The conservation value of these populations is highlighted by numerous studies documenting the erosion of native honeybee diversity through introgression and large-scale queen movements across Europe [25,267,282,283,284,285]. Population genetic analyses have revealed extensive admixture in several regions and a progressive reduction in the genetic integrity of some endemic populations, particularly A. mellifera [286,287]. These observations illustrate how directional breeding and unrestricted gene flow may inadvertently contribute to the loss of locally adapted genetic resources. Because gene flow among colonies is largely mediated through DCAs, the preservation of mating connectivity across landscapes may be as important as the preservation of colonies themselves. Conservation strategies may therefore benefit from considering not only the protection of locally adapted populations but also the maintenance of the mating structures that sustain population-level genetic exchange.
These populations collectively represent an immense reservoir of adaptive variation that cannot be fully captured by any single breeding programme [288,289,290]. Importantly, these locally adapted populations represent adaptive solutions already tested by natural selection under diverse ecological conditions, providing a complementary source of innovation to that generated by artificial breeding programmes.
From an evolutionary perspective, conservation therefore serves a function that extends beyond the preservation of subspecies or historical lineages. Conservation maintains alternative adaptive strategies, rare alleles, locally adapted gene complexes, and evolutionary trajectories that may become valuable under future environmental conditions. At the same time, breeding transforms part of this diversity into immediate gains in colony performance and management suitability. The two processes are therefore complementary: conservation maintains adaptive possibilities, whereas breeding exploits part of those possibilities to address present needs.
Rather than viewing conservation and breeding as competing objectives, it may be more useful to consider them as different expressions of adaptive population management operating at different points along a continuum of selection intensity. Such a perspective allows current productivity and future evolutionary resilience to be pursued simultaneously. The challenge then becomes not whether populations should be selected, but how different levels of artificial and natural selection can be organized to maximize both immediate performance and long-term adaptive potential.
A second level consists of conservation populations managed to preserve the genetic integrity and adaptive characteristics of native subspecies or regional ecotypes. Unlike sanctuary populations, conservation populations may involve active management, including controlled mating, monitoring of introgression, genomic characterization, and maintenance of effective population size.
The primary objective of these populations is to conserve evolutionary lineages and local adaptations while maintaining sufficient genetic diversity to avoid excessive inbreeding. Such programmes already exist for several subspecies of A. mellifera, including conservation initiatives for A. m. mellifera, A. m. ligustica, A. m. carnica, A. m. iberica, A. m. siciliana, A. m. caucasica and other locally adapted populations. Beyond preserving taxonomic diversity, these programmes contribute to the maintenance of adaptive variation generated through long-term interactions between populations and their environments. Examples of conservation programmes and protected populations of A. mellifera across Europe and the Mediterranean region. These initiatives illustrate a range of approaches, including protected conservation areas, controlled mating systems, genomic monitoring, conservation breeding, and international conservation networks. Collectively, they aim to preserve locally adapted genetic resources while maintaining the evolutionary potential necessary for future adaptation [290].
6.5. An Integrated Conservation–Breeding Framework for Adaptive Honeybee Improvement
The preceding sections suggest that neither intensive artificial selection nor the complete absence of management alone is sufficient to ensure the long-term sustainability of honeybee populations. While intensive breeding can accelerate genetic gain, it may progressively reduce genetic diversity and adaptive flexibility. Conversely, populations evolving exclusively under natural selection preserve evolutionary processes but do not necessarily satisfy the economic and management requirements of modern apiculture.
Rather than considering conservation and breeding as opposing strategies, we propose an integrated population-based framework in which different populations perform complementary evolutionary functions. The objective is not simply to improve colony performance, but to organise the continuous capture, preservation, and transfer of adaptive variation from naturally evolving populations toward economically valuable breeding populations.
Within this framework, natural selection continuously generates and filters adaptive variation, conservation populations preserve this diversity, breeding populations amplify desirable traits while maintaining broad genetic diversity, and dedicated crossing populations convert improved pure strains into commercial stocks.
Selection intensity therefore increases progressively across four spatially separated population types, each associated with independent mating systems and specific breeding objectives (Figure 6).
6.5.1. Natural Evolutionary Sanctuaries
The first component consists of sanctuary populations maintained under little or no intentional human selection. These populations may include feral colonies, isolated native populations, or protected conservation areas in which colony survival depends almost entirely on natural selection.
Their objective is not to maximize productivity but to maintain ongoing evolutionary processes. Natural mating, swarming, competition, predation, parasites, pathogens and local environmental conditions continuously generate and filter adaptive variation. These populations therefore constitute the primary evolutionary engine of the entire breeding system.
Unlike conventional breeding populations, sanctuary populations are not managed to produce superior colonies. Instead, they generate novel adaptive combinations that may subsequently become valuable under future environmental conditions.
6.5.2. Conservation Populations
The second component consists of protected conservation populations sharing the same mating network (DCA) as sanctuary populations. Their objective is to preserve the genetic integrity of locally adapted subspecies while allowing natural evolutionary processes to continue. Human intervention remains minimal and is restricted to preventing introgression, removing obvious hybrids or severely diseased colonies, and maintaining sufficient effective population size. Because these populations remain genetically connected to sanctuary populations, they preserve not only existing diversity but also the adaptive variation continuously generated by natural selection. Importantly, these populations also constitute the genetic source from which breeding material is periodically sampled.
6.5.3. Adaptive Within-Strain Breeding Populations
Adaptive breeding populations represent the interface between conservation and genetic improvement. Rather than introducing external genetic material, larvae or queens are periodically obtained from conservation populations and transferred into dedicated breeding areas possessing their own isolated mating system. The objective is to improve economically important traits while maintaining the genetic identity of the original subspecies.
Selection is based primarily on mass selection operating at the population level. Colonies exhibiting poor adaptation, low productivity, disease susceptibility or undesirable behavioural traits are progressively removed, whereas colonies combining favourable characteristics contribute proportionally more offspring to subsequent generations.
Unlike conventional breeding programmes that concentrate reproduction among a small number of elite colonies, this strategy maintains a broad breeding population, thereby preserving effective population size and reducing the loss of adaptive diversity.
Natural mating within isolated drone congregation areas remains the preferred method of reproduction. Instrumental insemination may occasionally be used for specific breeding objectives but should remain limited whenever possible in order to preserve the evolutionary properties associated with natural mating systems.
Thus, genetic gain results primarily from progressive changes in allele frequencies across the entire breeding population rather than from the intensive multiplication of a few exceptional colonies.
6.5.4. Innovation and Hybridisation Populations
The relative merits of selection within local populations (Zone 3, Figure 6) versus inter-racial hybridization (Zone 4, Figure 6) have been debated since the early development of scientific honeybee breeding. Ruttner [291] argued that neither approach is universally superior; rather, their value depends on the breeding objective. Selection within a geographical subspecies exploits the substantial genetic variation present among locally adapted populations while preserving adaptations to regional climates, floral resources, seasonal brood cycles, pathogens, and overwintering conditions. Such programmes can improve economically important traits—including honey production, colony development, disease resistance, and behaviour—while maintaining the adaptive genetic architecture shaped by natural selection. Their long-term success, however, depends on effective mating control, sufficiently large breeding populations, and continued management to preserve genetic diversity.
By contrast, inter-racial hybridization seeks to combine genetically differentiated populations to exploit heterosis and complementary trait combinations. F1 hybrids frequently exhibit increased colony vigour, rapid spring development, and improved honey production, making hybrid breeding attractive for commercial beekeeping. However, hybrid performance depends strongly on the parental combinations, heterosis is generally not maintained beyond the F1 generation, and subsequent generations often display greater phenotypic variability together with the reappearance of undesirable traits. Moreover, indiscriminate replacement of local populations by imported breeding stock may progressively erode locally adapted genetic diversity, reducing the evolutionary potential upon which future breeding ultimately depends.
While Ruttner [291] presented intra-racial selection and inter-racial hybridization as alternative breeding strategies, the breeding schemes we suggest can integrate both approaches within a hierarchical breeding framework (Figure 6 and Figure 7).
Rather than representing competing philosophies, conservation and recurrent selection within locally adapted populations provide the genetic foundation for subsequent hybrid development. Conservation populations maintain adaptive diversity and serve as long-term reservoirs of genetic variation from which superior pure breeding lines are continuously selected. These improved pure lines subsequently become parental stocks for controlled hybridization, allowing breeders to exploit heterosis while avoiding the genetic replacement of the original locally adapted populations. In this framework, conservation is no longer viewed as an endpoint separate from commercial breeding, but rather as the essential upstream component that continuously supplies improved breeding material for downstream innovation.
This integrated breeding pipeline requires appropriate spatial and genetic organisation. Conservation populations must remain reproductively protected to preserve local adaptation and maintain effective population size, whereas hybrid production should occur in dedicated breeding systems using controlled mating, such as isolated mating stations or instrumental insemination. At the landscape scale, this implies a territorial organisation of mating areas. Protected conservation zones maintain locally adapted populations under recurrent selection, while separate breeding zones are dedicated to the production and evaluation of commercial hybrids. Such regulatory separation, supported by geographic isolation and appropriate legislation governing queen importation and mating areas, allows innovation through hybrid breeding without compromising the long-term conservation of native genetic resources.
Consequently, hybrid breeding should not be regarded as an alternative to conservation-oriented selection, but rather as its downstream application within an integrated breeding strategy. Long-term genetic progress depends on maintaining diverse, locally adapted conservation populations that continuously generate improved pure breeding lines while preserving the adaptive genetic variation required to respond to future environmental, pathological, and production challenges. Under this framework, conservation, pure-line improvement, and hybrid breeding become complementary stages of a single breeding system, reconciling the historical dichotomy proposed by [291] with the objectives of modern honeybee breeding.
Such an organised breeding framework provides mutual benefits for both commercial beekeeping and biodiversity conservation. Beekeepers benefit from sustained access to genetically improved pure lines and high-performing commercial hybrids, whereas conservation programmes benefit from clear objectives, dedicated conservation populations, and the long-term maintenance of adaptive genetic diversity. Rather than competing for resources, breeding and conservation become interdependent components of a coordinated genetic management strategy.
This approach is particularly relevant throughout Europe, the Middle East, and Africa, which together constitute the native range and evolutionary centre of Apis mellifera. These regions harbour numerous subspecies and locally adapted ecotypes that represent irreplaceable reservoirs of evolutionary and functional diversity. Organising breeding programmes at regional or national scales—through protected conservation areas, recurrent within-subspecies selection, and dedicated hybrid production systems—would allow the sustainable exploitation of this diversity while safeguarding its long-term persistence. Such territorial organisation could simultaneously support commercial queen production, maintain the genetic integrity of native populations, reduce uncontrolled introgression from imported stocks, and preserve the evolutionary potential required to respond to future environmental, pathological, and climatic challenges.
7. Conclusions: Toward an Evolutionary Framework for Honeybee Improvement
Honeybee breeding differs fundamentally from the breeding of most domesticated species because colony phenotypes emerge from interactions among thousands of genetically diverse individuals operating within changing environmental and temporal contexts. Throughout this review, we have shown that honeybee phenotypes are shaped by the combined effects of intrinsic biological mechanisms, environmental heterogeneity, and temporal dynamics acting across multiple biological scales. Consequently, colony performance cannot be regarded as a fixed property of individual genotypes but rather as an emergent property of populations interacting with their environment through time.
These biological characteristics challenge breeding strategies based exclusively on controlled mating, intensive directional selection, and the propagation of a limited number of elite colonies. Although such approaches have demonstrated considerable success in improving economically important traits, they may progressively reduce the adaptive diversity upon which future genetic improvement ultimately depends.
We therefore propose that honeybee breeding should no longer be viewed solely as the optimisation of colony performance but as the management of adaptive populations. Within this evolutionary framework, natural selection, conservation, and artificial selection are not competing processes but complementary components of a single breeding strategy. Naturally evolving populations continuously generate and maintain adaptive variation; conservation populations preserve this diversity and its associated evolutionary processes; adaptive breeding populations capture and amplify economically valuable traits while maintaining broad genetic diversity; and dedicated crossing populations convert improved pure strains into commercial breeding stocks.
This framework transforms the relationship between conservation and breeding. Rather than functioning as isolated activities, conservation becomes the primary source of adaptive diversity supporting long-term genetic improvement, while breeding becomes the mechanism by which part of this diversity is progressively translated into agronomically valuable traits. In this way, natural selection itself becomes an integral component of the breeding programme rather than an external evolutionary force acting independently of it.
Such an approach may offer a more resilient strategy for honeybee improvement under accelerating environmental change. Climate change, emerging pathogens, habitat degradation, and changing agricultural practices continually modify the selective pressures experienced by honeybee populations. Because these future conditions cannot be predicted with certainty, the long-term objective of breeding should extend beyond maximizing present-day performance to maintaining the evolutionary capacity of populations to generate future adaptive solutions.
Ultimately, the greatest value of a honeybee population may lie not only in the performance of its best colonies, but in its capacity to continuously produce new generations of well-adapted colonies. Preserving this adaptive potential while progressively translating it into sustainable genetic improvement may represent one of the central challenges—and opportunities—for honeybee breeding in the twenty-first century.
Supplementary Materials
The following supporting information can be downloaded at the website of this paper posted on Preprints.org.
Abbreviations
The following abbreviations are used in this manuscript:
| DCA | Drone Congregation Area |
| GEI | Genotype-by-Environment Interaction |
| G×E×T | Genotype by Environment by Time Interactions |
| RR | Recombination Rate |
References
- Falconer, D.S. Introduction to quantitative genetics, 4th ed. ed.; Mackay, T.F.C., Ed.; Longman: Harlow, Essex, England, 1996. [Google Scholar]
- Wilson, E.O. The insect societies. In The insect societies; 1971. [Google Scholar]
- Beye, M.; Gattermeier, I.; Hasselmann, M.; Gempe, T.; Schioett, M.; Baines, J.F.; et al. Exceptionally high levels of recombination across the honey bee genome. Genome Res. 2006, 16(11), 1339–44. [Google Scholar] [CrossRef]
- Liu, H.; Zhang, X.; Huang, J.; Chen, J.-Q.; Tian, D.; Hurst, L.D.; et al. Causes and consequences of crossing-over evidenced via a high-resolution recombinational landscape of the honey bee. Genome Biol. 2015, 16(1), 15. [Google Scholar] [CrossRef]
- Wallberg, A.; Glemin, S.; Webster, M.T. Extreme recombination frequencies shape genome variation and evolution in the honeybee, Apis mellifera. PLoS Genet. 2015, 11(4), e1005189. [Google Scholar] [CrossRef]
- Beye, M.; Hasselmann, M.; Fondrk, M.K.; Page, R.E.; Omholt, S.W. The Gene csd Is the Primary Signal for Sexual Development in the Honeybee and Encodes an SR-Type Protein. Cell 2003, 114(4), 419–29. [Google Scholar] [CrossRef]
- Beye, M. The dice of fate: the csd gene and how its allelic composition regulates sexual development in the honey bee, Apis mellifera. BioEssays 2004, 26(10), 1131–9. [Google Scholar] [CrossRef]
- Bilodeau, L.; Avalos, A.; Danka, R.G. Genetic diversity of the complementary sex-determiner (csd) gene in two closed breeding stocks of Varroa -resistant honey bees. Apidologie 2020. [Google Scholar] [CrossRef]
- Kolics, É.; Parrag, T.; Házi, F.; Szepesi, K.; Heltai, B.; Mátyás, K.; et al. An Alternative, High Throughput Method to Identify Csd Alleles of the Honey Bee. Insects 2020, 11(8). [Google Scholar] [CrossRef]
- Koeniger, N.; Koeniger, G.; Pechhacker, H. The nearer the better? Drones (Apis mellifera) prefer nearer drone congregation areas. Insectes Sociaux 2005, 52(1), 31–5. [Google Scholar] [CrossRef]
- Baudry, E.; Solignac, M.; Garnery, L.; Gries, M.; Cornuet, J.; Koeniger, N. Relatedness among honeybees (Apis mellifera) of a drone congregation. Proc. R. Soc. Lond. Ser. B Biol. Sci. 1998, 265(1409), 2009–14. [Google Scholar] [CrossRef]
- Laidlaw, H.H.; Page, R.E. Polyandry in honey bees Apis mellifera: sperm utilization and intracolony genetic relationships. Genetics 1984, 108(4), 985–97. [Google Scholar] [CrossRef]
- Moritz, R.F.A. Intracolonial worker relationship and sperm competition in the honeybee (Apis mellifera L.). Experientia 1986, 42(4), 445–8. [Google Scholar] [CrossRef]
- Franck, P.; Coussy, H.; Le Conte, Y.; Solignac, M.; Garnery, L.; Cornuet, J.-M. Microsatellite analysis of sperm admixture in honeybee. Insect Mol. Biol. 1999, 8(3), 419–21. [Google Scholar] [CrossRef]
- Franck, P.; Solignac, M.; Vautrin, D.; Cornuet, J.-M.; Koeniger, G.; Koeniger, N. Sperm competition and last-male precedence in the honeybee. Anim. Behav. 2002, 64(3), 503–9. [Google Scholar] [CrossRef]
- Schlüns, H.; Koeniger, G.; Koeniger, N.; Moritz, R.F.A. Sperm utilization pattern in the honeybee (Apis mellifera). Behav. Ecol. Sociobiol. 2004, 56(5), 458–63. [Google Scholar] [CrossRef]
- Koeniger, G.; Koeniger, N.; Ellis, J.; Connor, L.J. Mating Biology of Honey Bees (Apis mellifera); Wicwas Press LLC: Kalamazoo, MI, 2014; p. 155 p. [Google Scholar]
- Gençer, H.V.; Kahya, Y. Sperm competition in honey bees (Apis mellifera L.): the role of body size dimorphism in drones. Apidologie 2020, 51(1), 1–17. [Google Scholar] [CrossRef]
- Robert E. Page, J. Sperm Utilization in Social Insects. Annu. Rev. Entomol. 1986, 31(1), 297–320. [Google Scholar] [CrossRef]
- Rothenbuhler, W.C. Behavior genetics of nest cleaning in honey bees. IV. Responses of F1 and backcross generations to disease-killed brood. Am. Zool. 1964, 4(2), 111–23. [Google Scholar] [CrossRef]
- Robinson, G.E.; Page, R.E. Genetic determination of nectar foraging, pollen foraging, and nest-site scouting in honey bee colonies. Behav. Ecol. Sociobiol. 1989, 24(5), 317–23. [Google Scholar] [CrossRef]
- Winston, M.L. The biology of the honey bee; Harvard University Press: Cambridge, Mass, 1991. [Google Scholar]
- Seeley, T.D. Honeybee democracy; Princeton University Press, 2010. [Google Scholar]
- Ruttner, F. Biogeography and Taxonomy of Honeybees1988.
- Requier, F.; Garnery, L.; Kohl, P.L.; Njovu, H.K.; Pirk, C.W.W.; Crewe, R.M.; et al. The conservation of native honey bees is crucial. Trends Ecol. Evol. 2019, 34(9), 789–98. [Google Scholar] [CrossRef]
- Li, W.; Freudenberg, J. Two-parameter characterization of chromosome-scale recombination rate. Genome Res. 2009, 19(12), 2300–7. [Google Scholar] [CrossRef]
- Wilfert, L.; Gadau, J.; Schmid-Hempel, P. Variation in genomic recombination rates among animal taxa and the case of social insects. Heredity 2007, 98(4), 189–97. [Google Scholar] [CrossRef]
- Meznar, E.R.; Gadau, J.; Koeniger, N.; Rueppell, O. Comparative Linkage Mapping Suggests a High Recombination Rate in All Honeybees. J. Hered. 2010, 101 (Supplement 1), S118–S26. [Google Scholar] [CrossRef]
- Kent, C.F.; Minaei, S.; Harpur, B.A.; Zayed, A. Recombination is associated with the evolution of genome structure and worker behavior in honey bees. Proc. Natl. Acad. Sci. 2012, 109(44), 18012–7. [Google Scholar] [CrossRef]
- Bessoltane, N.; Toffano-Nioche, C.; Solignac, M.; Mougel, F. Fine Scale Analysis of Crossover and Non-Crossover and Detection of Recombination Sequence Motifs in the Honeybee (Apis mellifera). PLoS ONE 2012, 7(5), e36229. [Google Scholar] [CrossRef]
- Dzierzon, J. Papers on fertilization and parthenogenesis in the honey-bee. Eichstaidt Bienen-Ztg. 1845, 1–32. [Google Scholar]
- Hunt, G.J.; Page, R.E., Jr. Linkage analysis of sex determination in the honey bee (Apis mellifera). Mol. Gen. Genet. 1994, 244(5), 512–8. [Google Scholar] [CrossRef]
- Laidlaw, H.H.; Page, R.E. Mating designs. Bee Genet. Breed. 1986, 323, 344. [Google Scholar]
- Moritz, R.; Southwick, E.E. Bees as superorganisms: an evolutionary reality; Springer Science & Business Media, 1992. [Google Scholar]
- Laidlaw, H.H.; Page, R.E. Queen rearing and bee breeding1997. [CrossRef]
- Ruttner, F.; Mackensen, O. The Genetics of the Honeybee. Bee World 1952, 33(5), 71–9. [Google Scholar] [CrossRef]
- Woyke, J. Drone Larvae from Fertilized Eggs of the Honeybee. J. Apic. Res. 1963, 2(1), 19–24. [Google Scholar] [CrossRef]
- Beye, M.; Moritz, R.F.; Epplen, C. Sex linkage in the honeybee Apis mellifera detected by multilocus DNA fingerprinting. Naturwissenschaften 1994, 81(10), 460–2. [Google Scholar] [CrossRef]
- Hasselmann, M.; Fondrk, M.K.; Page, R.E.; Beye, M. Fine scale mapping in the sex locus region of the honey bee (Apis mellifera). Insect Mol. Biol. 2001, 10(6), 605–8. [Google Scholar] [CrossRef]
- Kaskinova, M.D.; Nikolenko, A.G. csd gene of honeybee: Genetic structure, functioning, and evolution. Russ. J. Genet. 2017, 53(3), 297–301. [Google Scholar] [CrossRef]
- Otte, M.; Netschitailo, O.; Weidtkamp-Peters, S.; Seidel, C.A.M.; Beye, M. Recognition of polymorphic Csd proteins determines sex in the honeybee. Sci. Adv. 2023, 9(40), eadg4239. [Google Scholar] [CrossRef]
- Lechner, S.; Ferretti, L.; Schöning, C.; Kinuthia, W.; Willemsen, D.; Hasselmann, M. Nucleotide Variability at Its Limit? Insights into the Number and Evolutionary Dynamics of the Sex-Determining Specificities of the Honey Bee Apis mellifera. Mol. Biol. Evol. 2014, 31(2), 272–87. [Google Scholar] [CrossRef]
- Zareba, J.; Blazej, P.; Laszkiewicz, A.; Sniezewski, L.; Majkowski, M.; Janik, S.; et al. Uneven distribution of complementary sex determiner (csd) alleles in Apis mellifera population. Sci. Rep. 2017, 7(1), 2317. [Google Scholar] [CrossRef]
- Page, R.E.; Erickson, E. H., Jr. Reproduction by Worker Honey Bees (Apis mellifera L.). Behav. Ecol. Sociobiol. 1988, 23(2), 117–26. [Google Scholar] [CrossRef]
- Visscher, P.K. A Quantitative Study of Worker Reproduction in Honey Bee Colonies. Behav. Ecol. Sociobiol. 1989, 25(4), 247–54. [Google Scholar] [CrossRef]
- Gençer, H.V.; Firatli, Ç. Reproductive and morphological comparisons of drones reared in queenright and laying worker colonies. J. Apic. Res. 2005, 44(4), 163–7. [Google Scholar] [CrossRef]
- Zaitoun, S.; Al-Majeed Al-Ghzawi, A.; Kridli, R. Monthly changes in various drone characteristics of Apis mellifera ligustica and Apis mellifera syriaca. Entomol. Sci. 2009, 12(2), 208–14. [Google Scholar] [CrossRef]
- Woyke, J. Increased food supply to all larvae after dequeening honey bee colonies. J. Apic. Res. 1999, 38(3-4), 117–23. [Google Scholar] [CrossRef]
- Mazeed, A.M. Morphometry and number of spermatozoa in drone honeybees (Hymenoptera: Apidae) reared under different conditions. Eur. J. Entomol. 2011, 108(4), 673. [Google Scholar] [CrossRef]
- Gençer, H.V.; Woyke, J. Eggs from Apis mellifera caucasica laying workers are larger than from queens. J. Apic. Res. 2006, 45, 173–9. [Google Scholar] [CrossRef]
- Stürup, M.; Baer-Imhoof, B.; Nash, D.R.; Boomsma, J.J.; Baer, B. When every sperm counts: factors affecting male fertility in the honeybee Apis mellifera. Behav. Ecol. 2013, 24(5), 1192–8. [Google Scholar] [CrossRef]
- Czekońska, K.; Chuda-Mickiewicz, B.; Samborski, J. Quality of honeybee drones reared in colonies with limited and unlimited access to pollen. Apidologie 2015, 46(1), 1–9. [Google Scholar] [CrossRef]
- Nguyen, V. Effects of protein nutrition and pollen supplementation of honeybee (Apis mellifera L.) colonies on characteristics of drones with particular reference to sexual maturity. MSc (Honours) thesis, University of Western Sydney, Hawkesbury, NSW, Australia, 1995. [Google Scholar]
- Rangel, J.; Fisher, A. Factors affecting the reproductive health of honey bee (Apis mellifera) drones—a review. Apidologie 2019, 50(6), 759–78. [Google Scholar] [CrossRef]
- Schlüns, H.; Schlüns, E.A.; van Praagh, J.; Moritz, R.F.A. Sperm numbers in drone honeybees (Apis mellifera) depend on body size. Apidologie 2003, 34(6), 577–84. [Google Scholar] [CrossRef]
- Graham, J.M.; Langstroth, L.L.; Dadant & Sons. The Hive and the honey bee: a new book on beekeeping which continues the tradition of Langstroth on the hive and the honeybee. Revised edition; Dadant & Sons: Hamilton, Illinois, 2015; Volume xxvi, p. 1057 pages p. [Google Scholar]
- Koeniger, N.; Koeniger, G.; Gries, M.; Tingek, S. Drone competition at drone congregation areas in four Apis species. Apidologie 2005, 36(2), 211–21. [Google Scholar] [CrossRef]
- Reyes, M.; Crauser, D.; Prado, A.; Le Conte, Y. Flight activity of honey bee (Apis mellifera) drones. Apidologie 2019, 50(5), 669–80. [Google Scholar] [CrossRef]
- Amiri, E.; Strand, M.K.; Rueppell, O.; Tarpy, D.R. Queen Quality and the Impact of Honey Bee Diseases on Queen Health: Potential for Interactions between Two Major Threats to Colony Health. Insects 2017, 8(2). [Google Scholar] [CrossRef]
- Moritz, R.F.A.; Lattorff, H.M.G.; Neumann, P.; Kraus, F.B.; Radloff, S.E.; Hepburn, H.R. Rare royal families in honeybees, Apis mellifera. Naturwissenschaften 2005, 92(10), 488–91. [Google Scholar] [CrossRef]
- Kraus, F.B.; Neumann, P.; Moritz, R.F.A. Genetic variance of mating frequency in the honeybee (Apis mellifera L.). Insectes Sociaux 2005, 52(1), 1–5. [Google Scholar] [CrossRef]
- Delaney, D.A.; Keller, J.J.; Caren, J.R.; Tarpy, D.R. The physical, insemination, and reproductive quality of honey bee queens (Apis mellifera L.). Apidologie 2011, 42(1), 1–13. [Google Scholar] [CrossRef]
- Woyke, J. Natural and Artificial Insemination of Queen Honeybees. Bee World 1962, 43(1), 21–5. [Google Scholar] [CrossRef]
- Al-Lawati, H.; Bienefeld, K. Maternal Age Effects on Embryo Mortality and Juvenile Development of Offspring in the Honey Bee (Hymenoptera: Apidae). Ann. Entomol. Soc. Am. 2009, 102(5), 881–8. [Google Scholar] [CrossRef]
- Baer, B.; Collins, J.; Maalaps, K.; den Boer, S.P.A. Sperm use economy of honeybee (Apis mellifera) queens. Ecol. Evol. 2016, 6(9), 2877–85. [Google Scholar] [CrossRef]
- Brodschneider, R.; Arnold, G.; Hrassnigg, N.; Crailsheim, K. Does Patriline Composition Change over a Honey Bee Queen’s Lifetime? Insects 2012, 3(3), 857–69. [Google Scholar] [CrossRef]
- Tarpy, D.R.; Nielsen, D.I. Sampling Error, Effective Paternity, and Estimating the Genetic Structure of Honey Bee Colonies (Hymenoptera: Apidae). Ann. Entomol. Soc. Am. 2002, 95(4), 513–28. [Google Scholar] [CrossRef]
- Withrow, J.M.; Tarpy, D.R. Cryptic “royal” subfamilies in honey bee (Apis mellifera) colonies. PLoS ONE 2018, 13(7), e0199124. [Google Scholar] [CrossRef]
- Page, R.E.; Robinson, G.E. The Genetics of Division of Labour in Honey Bee Colonies. In Advances in Insect Physiology; Evans, P.D., Ed.; Academic Press: 23, 1991; pp. 117–69. [Google Scholar]
- Oxley, P.R.; Oldroyd, B.P. The Genetic Architecture of Honeybee Breeding. In Advances in Insect Physiology. Advances in Insect Physiology.; Academic Press: 39, 2010; pp. 83–118. [Google Scholar]
- Page, R.E.; Robinson, G.E.; Fondrk, M.K.; Nasr, M.E. Effects of worker genotypic diversity on honey bee colony development and behavior (Apis mellifera L.). Behav. Ecol. Sociobiol. 1995, 36(6), 387–96. [Google Scholar] [CrossRef]
- Robinson, G.E. Regulation of division of labor in insect societies. Annu Rev. Entomol. 1992, 37(1), 637–65. [Google Scholar] [CrossRef]
- Seeley, T.D. The Wisdom of the Hive.
- The Social Physiology of Honey Bee Colonies; London, England, 1995.
- Lattorff, H.M.G.; Moritz, R.F.A. Genetic underpinnings of division of labor in the honeybee (Apis mellifera). Trends Genet. 2013, 29(11), 641–8. [Google Scholar] [CrossRef]
- Harpur, B.A.; Kent, C.F.; Molodtsova, D.; Lebon, J.M.D.; Alqarni, A.S.; Owayss, A.A.; et al. Population genomics of the honey bee reveals strong signatures of positive selection on worker traits. Proc. Natl. Acad. Sci. 2013, 111(7), 2614–9. [Google Scholar] [CrossRef]
- Getz, W.M.; Brückner, D.; Parisian, T.R. Kin structure and the swarming behavior of the honey bee Apis mellifera. Behav. Ecol. Sociobiol. 1982, 10(4), 265–70. [Google Scholar] [CrossRef]
- Page, R.E.; Robinson, G.E.; Fondrk, M.K. Genetic specialists, kin recognition and nepotism in honey-bee colonies. Nature 1989, 338(6216), 576–9. [Google Scholar] [CrossRef]
- Carlin, N.F.; Frumhoff, P.C. Nepotism in the honey bee. Nat. UK 1990, 346(6286), 706–7. [Google Scholar] [CrossRef]
- Mateo, J.M. Kin-recognition abilities and nepotism as a function of sociality. Proc. R. Soc. Lond. Ser. B Biol. Sci. 2002, 269(1492), 721–7. [Google Scholar] [CrossRef]
- Inbar, S.; Cohen, P.; Yahav, T.; Privman, E. Comparative study of population genomic approaches for mapping colony-level traits. PLoS Comput. Biol. 2020, 16(3), e1007653. [Google Scholar] [CrossRef]
- Eynard, S.E.; Vignal, A.; Basso, B.; Canale-Tabet, K.; Le Conte, Y.; Decourtye, A.; et al. Reconstructing queen genotypes by pool sequencing colonies in eusocial insects: statistical methods and their application to honeybee. Mol. Ecol. Resour. 2022. [Google Scholar] [CrossRef]
- Cremer, S.; Armitage, S.A.O.; Schmid-Hempel, P. Social Immunity. Curr. Biol. 2007, 17(16), R693–R702. [Google Scholar] [CrossRef]
- Johnson, B.R. Division of labor in honeybees: form, function, and proximate mechanisms. Behav. Ecol. Sociobiol. 2010, 64(3), 305–16. [Google Scholar] [CrossRef]
- Grozinger, C.M.; Sharabash, N.M.; Whitfield, C.W.; Robinson, G.E. Pheromone-mediated gene expression in the honey bee brain. Proc. Natl. Acad. Sci. 2003, 100 (suppl_2), 14519–25. [Google Scholar] [CrossRef]
- Grozinger, C.M.; Fan, Y.; Hoover, S.E.R.; Winston, M.L. Genome-wide analysis reveals differences in brain gene expression patterns associated with caste and reproductive status in honey bees (Apis mellifera). Mol. Ecol. 2007, 16(22), 4837–48. [Google Scholar] [CrossRef]
- Le Conte, Y.; Mohammedi, A.; Robinson, G.E. Primer effects of a brood pheromone on honeybee behavioural development. Proc. R. Soc. Lond. Ser. B Biol. Sci. 2001, 268(1463), 163–8. [Google Scholar] [CrossRef]
- Alaux, C.; Le Conte, Y.; Adams, H.; Rodriguez-Zas, S.; Grozinger, C.; Sinha, S.; et al. Regulation of brain gene expression in honey bees by brood pheromone. Genes Brain Behav. 2009, 8(3), 309–19. [Google Scholar] [CrossRef]
- Robinson, G.E.; Grozinger, C.M.; Whitfield, C.W. Sociogenomics: social life in molecular terms. Nat. Rev. Genet. 2005, 6(4), 257–70. [Google Scholar] [CrossRef]
- Holldobler, B.; Wilson, E.O. The superorganism: the beauty elegance and strangeness of insect societies; WW Norton & Company, 2009. [Google Scholar]
- Seeley, T.D.; Tarpy, D.R. Queen promiscuity lowers disease within honeybee colonies. Proc. Biol. Sci. 2007, 274(1606), 67–72. [Google Scholar] [CrossRef]
- Moritz, R.F.; Crozier, R.H.; Pamilo, P. (Eds.) Sociogenetics in insects: introduction. In Chemistry and biology of social insects: proceedings of the 10th international congress; München, 1987. [Google Scholar]
- Adam, B. search of the best strains of bees; Northern Bee Books, 1983. [Google Scholar]
- Döke, M.A.; Frazier, M.; Grozinger, C.M. Overwintering honey bees: biology and management. Curr. Opin. Insect Sci. 2015, 10, 185–93. [Google Scholar] [CrossRef]
- Richard, F.J.; Tarpy, D.R.; Grozinger, C.M. Effects of insemination quantity on honey bee queen physiology. PLoS ONE 2007, 2(10), e980. [Google Scholar] [CrossRef]
- Crozier, R.H.; Pamilo, P. Evolution of social insect colonies; Oxford University, 1996. [Google Scholar]
- Page, R.E., Jr. The evolution of multiple mating behavior by honey bee queens (Apis mellifera L.). Genetics 1980, 96(1), 263–73. [Google Scholar] [CrossRef]
- Ratnieks, F.W. The evolution of polyandry by queens in social Hymenoptera: the significance of the timing of removal of diploid males. Behav. Ecol. Sociobiol. 1990, 26(5), 343–8. [Google Scholar] [CrossRef]
- Tarpy, D.; Page, R. Sex determination and the evolution of polyandry in honey bees ( Apis mellifera ). Behav. Ecol. Sociobiol. 2002, 52(2), 143–50. [Google Scholar] [CrossRef]
- Dreller, C. Division of labor between scouts and recruits: genetic influence and mechanisms. Behav. Ecol. Sociobiol. 1998, 43(3), 191–6. [Google Scholar] [CrossRef]
- Kolmes, S.A.; Winston, M.L.; Fergusson, L.A. The Division of Labor among Worker Honey Bees (Hymenoptera: Apidae): The Effects of Multiple Patrilines. J. Kans. Entomol. Soc. 1989, 62(1), 80–95. [Google Scholar]
- Mattila, H.R.; Seeley, T.D. Extreme polyandry improves a honey bee colony’s ability to track dynamic foraging opportunities via greater activity of inspecting bees. Apidologie 2013, 45(3), 347–63. [Google Scholar] [CrossRef]
- Oldroyd, B.; Rinderer, T.; Buco, S. Intra-colonial foraging specialism by honey bees (Apis mellifera) (Hymenoptera:Apidae). Behav. Ecol. Sociobiol. 1992, 30(5), 291–5. [Google Scholar] [CrossRef]
- Oldroyd, B.P.; Rinderer, T.E.; Schwenke, J.R.; Buco, S.M. Subfamily recognition and task specialisation in honey bees (Apis mellifera L.) (Hymenoptera: Apidae). Behav. Ecol. Sociobiol. 1994, 34(3), 169–73. [Google Scholar] [CrossRef]
- Robinson, G.E.; Page, R.E. Genetic determination of guarding and undertaking in honey-bee colonies. Nature 1988, 333(6171), 356–8. [Google Scholar] [CrossRef]
- Robinson, G.E.; Page, R. Genetic basis for division of labor in an insect society. In The genetics of social evolution; 1989; pp. 61–80. [Google Scholar]
- Jones, J.C.; Myerscough, M.R.; Graham, S.; Oldroyd, B.P. Honey bee nest thermoregulation: diversity promotes stability. Science 2004, 305(5682), 402–4. [Google Scholar] [CrossRef]
- Oldroyd, B.P.; Fewell, J.H. Genetic diversity promotes homeostasis in insect colonies. Trends Ecol. Evol. 2007, 22(8), 408–13. [Google Scholar] [CrossRef]
- Carr-Markell, M.K.; McDonald, K.M.; Mattila, H.R. Intracolonial genetic diversity increases chemical signaling by waggle-dancing honey bees, Apis mellifera. Insectes Sociaux 2013, 60(4), 485–96. [Google Scholar] [CrossRef]
- Mattila, H.R.; Burke, K.M.; Seeley, T.D. Genetic diversity within honeybee colonies increases signal production by waggle-dancing foragers. Proc. Biol. Sci. 2008, 275(1636), 809–16. [Google Scholar] [CrossRef]
- Mattila, H.R.; Seeley, T.D. Does a polyandrous honeybee queen improve through patriline diversity the activity of her colony’s scouting foragers? Behav. Ecol. Sociobiol. 2011, 65(4), 799–811. [Google Scholar] [CrossRef]
- Hamilton, W. Kinship, recognition, disease, and intelligence: constraints of social evolution. Anim. Soc. Theor. Facts 1987, 81–100. [Google Scholar]
- Palmer, K.A.; Oldroyd, B.P. Evidence for intra-colonial genetic variance in resistance to American foulbrood of honey bees ( Apis mellifera): further support for the parasite/pathogen hypothesis for the evolution of polyandry. Naturwissenschaften 2003, 90(6), 265–8. [Google Scholar] [CrossRef]
- Schmid-Hempel, P. Parasites in social insects; Princeton University Press, 1998. [Google Scholar]
- Sherman, P.W.; Seeley, T.D.; Reeve, H.K. Parasites, Pathogens, and Polyandry in Social Hymenoptera. Am. Nat. 1988, 131(4), 602–10. [Google Scholar] [CrossRef]
- Tarpy, D.R. Genetic diversity within honeybee colonies prevents severe infections and promotes colony growth. Proc. Biol. Sci. 2003, 270(1510), 99–103. [Google Scholar] [CrossRef]
- Tarpy, D.R.; Seeley, T.D. Lower disease infections in honeybee (Apis mellifera) colonies headed by polyandrous vs monandrous queens. Naturwissenschaften 2006, 93(4), 195–9. [Google Scholar] [CrossRef]
- Wilson-Rich, N.; Spivak, M.; Fefferman, N.H.; Starks, P.T. Genetic, individual, and group facilitation of disease resistance in insect societies. Annu Rev. Entomol. 2009, 54(1), 405–23. [Google Scholar] [CrossRef]
- Eckholm, B.J.; Anderson, K.E.; Weiss, M.; DeGrandi-Hoffman, G. Intracolonial genetic diversity in honeybee (Apis mellifera) colonies increases pollen foraging efficiency. Behav. Ecol. Sociobiol. 2011, 65(5), 1037–44. [Google Scholar] [CrossRef]
- Kraus, F.B.; Gerecke, E.; Moritz, R.F. Shift work has a genetic basis in honeybee pollen foragers (Apis mellifera L.). Behav. Genet. 2011, 41(2), 323–8. [Google Scholar] [CrossRef]
- Lobo, J.A.; Kerr, W.E. Estimation of the number of matings inApis mellifera: extensions of the model and comparison of different estimates. Ethol. Ecol. Evol. 1993, 5(3), 337–45. [Google Scholar] [CrossRef]
- Tarpy, D.R.; Vanengelsdorp, D.; Pettis, J.S. Genetic diversity affects colony survivorship in commercial honey bee colonies. Naturwissenschaften 2013, 100(8), 723–8. [Google Scholar] [CrossRef]
- Vanengelsdorp, D.; Meixner, M.D. A historical review of managed honey bee populations in Europe and the United States and the factors that may affect them. J. Invertebr. Pathol. 2010, 103 Suppl 1, S80–95. [Google Scholar] [CrossRef]
- Fuchs, S.; Moritz, R.F.A. Evolution of extreme polyandry in the honeybee Apis mellifera L. Behav. Ecol. Sociobiol. 1999, 45(3-4), 269–75. [Google Scholar] [CrossRef]
- Mattila, H.R.; Seeley, T.D. Genetic diversity in honey bee colonies enhances productivity and fitness. Science 2007, 317(5836), 362–4. [Google Scholar] [CrossRef]
- Steinhauer, N.; Vanengelsdorp, D.; Saegerman, C. Prioritizing changes in management practices associated with reduced winter honey bee colony losses for US beekeepers. Sci. Total Environ. 2021, 753, 141629. [Google Scholar] [CrossRef]
- Harpur, B.A.; Minaei, S.; Kent, C.F.; Zayed, A. Management increases genetic diversity of honey bees via admixture. Mol. Ecol. 2012, 21(18), 4414–21. [Google Scholar] [CrossRef]
- Tarpy, D.R.; Hatch, S.; Fletcher, D.J.C. The influence of queen age and quality during queen replacement in honeybee colonies. Anim. Behav. 2000, 59(1), 97–101. [Google Scholar] [CrossRef]
- Simone-Finstrom, M.; Li-Byarlay, H.; Huang, M.H.; Strand, M.K.; Rueppell, O.; Tarpy, D.R. Migratory management and environmental conditions affect lifespan and oxidative stress in honey bees. Sci. Rep. 2016, 6(1), 32023. [Google Scholar] [CrossRef]
- Nolan, M.P.; Delaplane, K.S. Distance between honey bee Apis mellifera colonies regulates populations of Varroa destructor at a landscape scale. Apidologie 2017, 48(1), 8–16. [Google Scholar] [CrossRef]
- Mortensen, A.N.; Jack, C.J.; Bustamante, T.A.; Schmehl, D.R.; Ellis, J.D. Effects of supplemental pollen feeding on honey bee (Hymenoptera: Apidae) colony strength and Nosema spp. infection. J. Econ. Entomol. 2019, 112(1), 60–6. [Google Scholar] [CrossRef]
- Ricigliano, V.A.; Williams, S.T.; Oliver, R. Effects of different artificial diets on commercial honey bee colony performance, health biomarkers, and gut microbiota. BMC Vet. Res. 2022, 18(1), 52. [Google Scholar] [CrossRef]
- van Dooremalen, C.; Gerritsen, L.; Cornelissen, B.; van der Steen, J.J.M.; van Langevelde, F.; Blacquière, T. Winter Survival of Individual Honey Bees and Honey Bee Colonies Depends on Level of Varroa destructor Infestation. PLoS ONE 2012, 7(4), e36285. [Google Scholar] [CrossRef]
- Jack, C.J.; Ellis, J.D. Integrated Pest Management Control of Varroa destructor (Acari: Varroidae), the Most Damaging Pest of (Apis mellifera L. (Hymenoptera: Apidae)) Colonies. J. Insect Sci. 2021, 21(5). [Google Scholar] [CrossRef]
- Gray, D.; Goslee, S.; Kammerer, M.; Grozinger, C.M. Effective pest management approaches can mitigate honey bee (Apis mellifera) colony winter loss across a range of weather conditions in small-scale, stationary apiaries. J. Insect Sci. 2024, 24(3). [Google Scholar] [CrossRef]
- Alaux, C.; Allier, F.; Decourtye, A.; Odoux, J.-F.; Tamic, T.; Chabirand, M.; et al. A ‘Landscape physiology’ approach for assessing bee health highlights the benefits of floral landscape enrichment and semi-natural habitats. Sci. Rep. 2017, 7(1), 40568. [Google Scholar] [CrossRef]
- St. Clair, A.L.; Zhang, G.; Dolezal, A.G.; O’Neal, M.E.; Toth, A.L. Diversified Farming in a Monoculture Landscape: Effects on Honey Bee Health and Wild Bee Communities. Environ. Entomol. 2020, 49(3), 753–64. [Google Scholar] [CrossRef]
- Mallinger, R.E.; Gaines-Day, H.R.; Gratton, C. Do managed bees have negative effects on wild bees?: A systematic review of the literature. PLoS ONE 2017, 12(12), e0189268. [Google Scholar] [CrossRef]
- Wojcik, V.A.; Morandin, L.A.; Davies Adams, L.; Rourke, K.E. Floral resource competition between honey bees and wild bees: is there clear evidence and can we guide management and conservation? Environ. Entomol. 2018, 47(4), 822–33. [Google Scholar] [CrossRef]
- Roberts, W.C.; Taber, S., 3RD. Egg-Weight Variance in Honey Bees. Ann. Entomol. Soc. Am. 1965, 58(3), 303–6. [Google Scholar] [CrossRef]
- Amiri, E.; Le, K.; Melendez, C.V.; Strand, M.K.; Tarpy, D.R.; Rueppell, O. Egg-size plasticity in Apis mellifera: Honey bee queens alter egg size in response to both genetic and environmental factors. J. Evol. Biol. 2020, 33(4), 534–43. [Google Scholar] [CrossRef]
- Fine, J.D.; Shpigler, H.Y.; Ray, A.M.; Beach, N.J.; Sankey, A.L.; Cash-Ahmed, A.; et al. Quantifying the effects of pollen nutrition on honey bee queen egg laying with a new laboratory system. PLoS ONE 2018, 13(9), e0203444. [Google Scholar] [CrossRef]
- Hejtmanek, J. O variabilite vc elich vajic ek. On the variability of the eggs of the honeybee. Ved. Pr. Vyzk. Ust. Vcelar CAZV V. Dole 1961, 169–96. [Google Scholar]
- Taber, S., 3rd; Roberts, W.C. Egg Weight Variability and its Inheritance in the Honey Bee. Ann. Entomol. Soc. Am. 1963, 56(4), 473–6. [Google Scholar] [CrossRef]
- Nelson, J.A. The embryology of the honey bee; Princeton University Press, 1915. [Google Scholar]
- Jay, S.C. The Development of Honeybees in their Cells. J. Apic. Res. 1963, 2(2), 117–34. [Google Scholar] [CrossRef]
- Doull, K.M. The Effects of Different Humidities on the Hatching of the Eggs of Honeybees. Apidologie 1976, 7(1), 61–6. [Google Scholar] [CrossRef]
- Al-Ghamdi, A.A.; Al-Khaibari, A.M.; Omar, M.O. Consumption rate of some proteinic diets affecting hypopharyngeal glands development in honeybee workers. Saudi J. Biol. Sci. 2011, 18(1), 73–7. [Google Scholar] [CrossRef]
- Hu, X.; Ke, L.; Wang, Z.; Zeng, Z. Dynamic transcriptome landscape of Asian domestic honeybee (Apis cerana) embryonic development revealed by high-quality RNA sequencing. BMC Dev. Biol. 2018, 18(1), 11. [Google Scholar] [CrossRef]
- Wegener, J.; Huang, Z.Y.; Lorenz, M.W.; Bienefeld, K. Regulation of hypopharyngeal gland activity and oogenesis in honey bee (Apis mellifera) workers. J. Insect Physiol. 2009, 55(8), 716–25. [Google Scholar] [CrossRef]
- Amiri, E.; Herman, J.J.; Strand, M.K.; Tarpy, D.R.; Rueppell, O. Egg transcriptome profile responds to maternal virus infection in honey bees, Apis mellifera. Infect. Genet. Evol. 2020, 85, 104558. [Google Scholar] [CrossRef]
- Salmela, H.; Amdam, G.V.; Freitak, D. Transfer of Immunity from Mother to Offspring Is Mediated via Egg-Yolk Protein Vitellogenin. PLoS Pathog. 2015, 11(7), e1005015. [Google Scholar] [CrossRef]
- Harwood, G.; Amdam, G.; Freitak, D. The role of Vitellogenin in the transfer of immune elicitors from gut to hypopharyngeal glands in honey bees (Apis mellifera). J. Insect Physiol. 2019, 112, 90–100. [Google Scholar] [CrossRef]
- Li, J.; Zhang, L.; Feng, M.; Zhang, Z.; Pan, Y. Identification of the proteome composition occurring during the course of embryonic development of bees (Apis mellifera). Insect Mol. Biol. 2009, 18(1), 1–9. [Google Scholar] [CrossRef]
- Nelson, J.A.; Sturtevant, A.P.; Lineburg, B. Growth and feeding of honeybee larvae: US Department of Agriculture; 1924. [Google Scholar]
- Thrasyvoulou, A.T.; Benton, A.W. Rates of Growth of Honeybee Larvae. J. Apic. Res. 1982, 21(4), 189–92. [Google Scholar] [CrossRef]
- Wirtz, P. Differentiation in the honeybee larva: a histological, electron-microscopical and physiological study of caste induction in Apis mellifera mellifera L.; Veenman: Wageningen, 1973. [Google Scholar]
- Bishop, G.H. Growth rates of honey bee larva. J. Exp. Zool. 1961, 146(1), 11–20. [Google Scholar] [CrossRef]
- Schnelle, H. Über den feineren bau des fettkörpers der honigbiene1923. [CrossRef]
- Wang, D.-I. Growth Rates of Young Queen and Worker Honeybee Larvae. J. Apic. Res. 1965, 4(1), 3–5. [Google Scholar] [CrossRef]
- Dietz, A.; Haydak, M.H. Caste determination in honey bees. I. The significane of moisture in larval food. J. Exp. Zool. 1971, 177(3), 353–7. [Google Scholar] [CrossRef]
- Ellis, M.B.; Nicolson, S.W.; Crewe, R.M.; Dietemann, V. Hygropreference and brood care in the honeybee (Apis mellifera). J. Insect Physiol. 2008, 54(12), 1516–21. [Google Scholar] [CrossRef]
- Zhu, K.; Liu, M.; Fu, Z.; Zhou, Z.; Kong, Y.; Liang, H.; et al. Plant microRNAs in larval food regulate honeybee caste development. PLoS Genet. 2017, 13(8), e1006946. [Google Scholar] [CrossRef]
- Slater, G.P.; Yocum, G.D.; Bowsher, J.H. Diet quantity influences caste determination in honeybees (Apis mellifera). Proc. Biol. Sci. 2020, 287(1927), 20200614. [Google Scholar] [CrossRef]
- Alhosin, M. Epigenetics Mechanisms of Honeybees: Secrets of Royal Jelly. Epigenet. Insights 2023, 16, 25168657231213717. [Google Scholar] [CrossRef]
- Alaux, C.; Ducloz, F.; Crauser, D.; Le Conte, Y. Diet effects on honeybee immunocompetence. Biol. Lett. 2010, 6(4), 562–5. [Google Scholar] [CrossRef]
- Di Pasquale, G.; Salignon, M.; Le Conte, Y.; Belzunces, L.P.; Decourtye, A.; Kretzschmar, A.; et al. Influence of pollen nutrition on honey bee health: do pollen quality and diversity matter? PLoS ONE 2013, 8(8), e72016. [Google Scholar] [CrossRef]
- Crailsheim, K. The flow of jelly within a honeybee colony. J. Comp. Physiol. B 1992, 162(8), 681–9. [Google Scholar] [CrossRef]
- DeGrandi-Hoffman, G.; Chen, Y.; Huang, E.; Huang, M.H. The effect of diet on protein concentration, hypopharyngeal gland development and virus load in worker honey bees (Apis mellifera L.). J. Insect Physiol. 2010, 56(9), 1184–91. [Google Scholar] [CrossRef]
- Alaux, C.; Dantec, C.; Parrinello, H.; Le Conte, Y. Nutrigenomics in honey bees: digital gene expression analysis of pollen’s nutritive effects on healthy and varroa-parasitized bees. BMC Genom. 2011, 12, 496. [Google Scholar] [CrossRef]
- Barascou, L.; Sene, D.; Barraud, A.; Michez, D.; Lefebvre, V.; Medrzycki, P.; et al. Pollen nutrition fosters honeybee tolerance to pesticides. R. Soc. Open Sci. 2021, 8(9), 210818. [Google Scholar] [CrossRef]
- Dolezal, A.G.; Toth, A.L. Feedbacks between nutrition and disease in honey bee health. Curr. Opin. Insect Sci. 2018, 26, 114–9. [Google Scholar] [CrossRef]
- DeGrandi-Hoffman, G.; Chen, Y. Nutrition, immunity and viral infections in honey bees. Curr. Opin. Insect Sci. 2015, 10, 170–6. [Google Scholar] [CrossRef]
- Donkersley, P.; Rhodes, G.; Pickup, R.W.; Jones, K.C.; Wilson, K. Honeybee nutrition is linked to landscape composition. Ecol. Evol. 2014, 4(21), 4195–206. [Google Scholar] [CrossRef]
- Di Pasquale, G.; Alaux, C.; Le Conte, Y.; Odoux, J.F.; Pioz, M.; Vaissiere, B.E.; et al. Variations in the Availability of Pollen Resources Affect Honey Bee Health. PLoS ONE 2016, 11(9), e0162818. [Google Scholar] [CrossRef]
- Brown, A.F.; Rodriguez, V.; Brzoska, C.; Pfister, J.; Neumann, P.; Retschnig, G. Dream Team for Honey Bee Health: Pollen and Unmanipulated Gut Microbiota Promote Worker Longevity and Body Weight. In Frontiers in Sustainable Food Systems; 2022; Volume 6 - 2022. [Google Scholar]
- Najarpoor, A.; Mohamadzade Namin, S.; Ghosh, S.; Jung, C. Impact of carbohydrate sources on the longevity and physiological traits of the European honey bee workers. Sci. Rep. 2025, 15(1), 29532. [Google Scholar] [CrossRef]
- Donkersley, P.; Rhodes, G.; Pickup, R.W.; Jones, K.C.; Power, E.F.; Wright, G.A.; et al. Nutritional composition of honey bee food stores vary with floral composition. Oecologia 2017, 185(4), 749–61. [Google Scholar] [CrossRef]
- Lee, K.V.; Goblirsch, M.; McDermott, E.; Tarpy, D.R.; Spivak, M. Is the Brood Pattern within a Honey Bee Colony a Reliable Indicator of Queen Quality? Insects 2019, 10(1), 12. [Google Scholar] [CrossRef]
- Avni, D.; Hendriksma, H.P.; Dag, A.; Uni, Z.; Shafir, S. Nutritional aspects of honey bee-collected pollen and constraints on colony development in the eastern Mediterranean. J. Insect Physiol. 2014, 69, 65–73. [Google Scholar] [CrossRef]
- Alburaki, M.; Steckel, S.J.; Williams, M.T.; Skinner, J.A.; Tarpy, D.R.; Meikle, W.G.; et al. Agricultural Landscape and Pesticide Effects on Honey Bee (Hymenoptera: Apidae) Biological Traits. J. Econ. Entomol. 2017, 110(3), 835–47. [Google Scholar] [CrossRef]
- Hatjina, F.; Costa, C.; Büchler, R.; Uzunov, A.; Drazic, M.; Filipi, J.; et al. Population dynamics of European honey bee genotypes under different environmental conditions. J. Apic. Res. 2014, 53(2), 233–47. [Google Scholar] [CrossRef]
- Quinlan, G.; Milbrath, M.; Otto, C.; Smart, A.; Iwanowicz, D.; Cornman, R.S.; et al. Honey bee foraged pollen reveals temporal changes in pollen protein content and changes in forager choice for abundant versus high protein flowers. Agric. Ecosyst. Environ. 2021, 322, 107645. [Google Scholar] [CrossRef]
- Brodschneider, R.; Crailsheim, K. Nutrition and health in honey bees. Apidologie 2010, 41(3), 278–94. [Google Scholar] [CrossRef]
- DeGrandi-Hoffman, G.; Chen, Y.; Rivera, R.; Carroll, M.; Chambers, M.; Hidalgo, G.; et al. Honey bee colonies provided with natural forage have lower pathogen loads and higher overwinter survival than those fed protein supplements. Apidologie 2016, 47(2), 186–96. [Google Scholar] [CrossRef]
- Bosco, L.; Yañez, O.; Schauer, A.; Maurer, C.; Cushman, S.A.; Arlettaz, R.; et al. Landscape structure affects temporal dynamics in the bumble bee virome: Landscape heterogeneity supports colony resilience. Sci. Total Environ. 2024, 946, 174280. [Google Scholar] [CrossRef]
- Maurer, C.; Schauer, A.; Yañez, O.; Neumann, P.; Gajda, A.; Paxton, R.J.; et al. Species traits, landscape quality and floral resource overlap with honeybees determine virus transmission in plant–pollinator networks. Nat. Ecol. Evol. 2024, 8(12), 2239–51. [Google Scholar] [CrossRef]
- Danner, N.; Keller, A.; Härtel, S.; Steffan-Dewenter, I. Honey bee foraging ecology: Season but not landscape diversity shapes the amount and diversity of collected pollen. PLoS ONE 2017, 12(8), e0183716. [Google Scholar] [CrossRef]
- Tsuruda, J.M.; Chakrabarti, P.; Sagili, R.R. Honey Bee Nutrition; Veterinary Clinics of North America: Food Animal Practice, 2021; Volume 37, 3, pp. 505–19. [Google Scholar]
- Hollands, G.; Snaddon, J.L.; Newland, P.L.; Sharkh, S.M. The impact of landscape complexity and composition on honey bee visual learning. J. Exp. Biol. 2025, 228(13). [Google Scholar] [CrossRef]
- Ricigliano, V.A.; Mott, B.M.; Floyd, A.S.; Copeland, D.C.; Carroll, M.J.; Anderson, K.E. Honey bees overwintering in a southern climate: longitudinal effects of nutrition and queen age on colony-level molecular physiology and performance. Sci. Rep. 2018, 8(1). [Google Scholar] [CrossRef]
- Mainardi, G.; Sponsler, D.; Minaud, E.; Vardakas, F.; Charistos, L.; Requier, F.; et al. Floral diversity enhances winter survival of honeybee colonies across climatic regions. J. Appl. Ecol. 2025, 62(6), 1487–97. [Google Scholar] [CrossRef]
- Dolezal, A.G.; St. Clair, A.L.; Zhang, G.; Toth, A.L.; O’Neal, M.E. Native habitat mitigates feast–famine conditions faced by honey bees in an agricultural landscape. Proc. Natl. Acad. Sci. 2019, 116(50), 25147–55. [Google Scholar] [CrossRef]
- Quinlan, G.M.; Grozinger, C.M. Chapter Five - Honey bee nutritional ecology: From physiology to landscapes. In Advances in Insect Physiology; Harrison, J.F., Ed.; Academic Press: 64, 2023; pp. 289–345. [Google Scholar]
- Motta, E.V.S.; Moran, N.A. The honeybee microbiota and its impact on health and disease. Nat. Rev. Microbiol. 2024, 22(3), 122–37. [Google Scholar] [CrossRef]
- Minaud, É.; Rebaudo, F.; Davidson, P.; Hatjina, F.; Hotho, A.; Mainardi, G.; et al. How stressors disrupt honey bee biological traits and overwintering mechanisms. Heliyon 2024, 10(14), e34390. [Google Scholar] [CrossRef]
- Minaud, E.; Rebaudo, F.; Mainardi, G.; Vardakas, P.; Hatjina, F.; Steffan-Dewenter, I.; et al. Temperature in overwintering honey bee colonies reveals brood status and predicts colony mortality. Ecol. Indic. 2024, 169, 112961. [Google Scholar] [CrossRef]
- Moritz, R.F. Nourishment and sociality in honeybees. In Nourishment and evolution in insect societies; Hunt, J.H., Nalepa, C.A., Eds.; Westview press: Boulder, CO, 1994; pp. 345–90. [Google Scholar]
- Wang, H.; Zhang, S.-W.; Zeng, Z.-J.; Yan, W.-Y. Nutrition affects longevity and gene expression in honey bee (Apis mellifera) workers. Apidologie 2014, 45(5), 618–25. [Google Scholar] [CrossRef]
- Zhang, Z.; Mu, X.; Shi, Y.; Zheng, H. Distinct roles of honeybee gut bacteria on host metabolism and neurological processes. Microbiol. Spectr. 2022, 10(2), e02438-21. [Google Scholar] [CrossRef]
- Cabirol, A.; Moriano-Gutierrez, S.; Engel, P. Neuroactive metabolites modulated by the gut microbiota in honey bees. Mol. Microbiol. 2024, 122(3), 284–93. [Google Scholar] [CrossRef]
- Liberti, J.; Kay, T.; Quinn, A.; Kesner, L.; Frank, E.T.; Cabirol, A.; et al. The gut microbiota affects the social network of honeybees. Nat. Ecol. Evol. 2022, 6(10), 1471–9. [Google Scholar] [CrossRef]
- Scheiner, R.; Page, R.E.; Erber, J. The Effects of Genotype, Foraging Role, and Sucrose Responsiveness on the Tactile Learning Performance of Honey Bees (Apis mellifera L.). Neurobiol. Learn. Mem. 2001, 76(2), 138–50. [Google Scholar] [CrossRef]
- Scheiner, R.; Page, R.E.; Erber, J. Sucrose responsiveness and behavioral plasticity in honey bees (Apis mellifera). Apidologie 2004, 35(2), 133–42. [Google Scholar] [CrossRef]
- Page, R.E., Jr.; Erber, J.; Fondrk, M.K. The effect of genotype on response thresholds to sucrose and foraging behavior of honey bees (Apis mellifera L.). J. Comp. Physiol. A 1998, 182(4), 489–500. [Google Scholar] [CrossRef]
- Page, R.E.; Erber, J. Levels of behavioral organization and the evolution of division of labor. Naturwissenschaften 2002, 89(3), 91–106. [Google Scholar] [CrossRef]
- Wang, Y.; Kaftanoglu, O.; Brent, C.S.; Page, R.E., Jr.; Amdam, G.V. Starvation stress during larval development facilitates an adaptive response in adult worker honey bees (Apis mellifera L.). J. Exp. Biol. 2016, 219(7), 949–59. [Google Scholar] [CrossRef]
- Toth, A.L.; Robinson, G.E. Worker nutrition and division of labour in honeybees. Anim. Behav. 2005, 69(2), 427–35. [Google Scholar] [CrossRef]
- Maes, P.W.; Rodrigues, P.A.P.; Oliver, R.; Mott, B.M.; Anderson, K.E. Diet-related gut bacterial dysbiosis correlates with impaired development, increased mortality and Nosema disease in the honeybee (Apis mellifera). Mol. Ecol. 2016, 25(21), 5439–50. [Google Scholar] [CrossRef]
- Kešnerová, L.; Emery, O.; Troilo, M.; Liberti, J.; Erkosar, B.; Engel, P. Gut microbiota structure differs between honeybees in winter and summer. ISME Journal. 2020, 14(3), 801–14. [Google Scholar] [CrossRef]
- Eckholm, B.J.; Huang, M.H.; Anderson, K.E.; Mott, B.M.; DeGrandi-Hoffman, G. Honey bee (Apis mellifera) intracolonial genetic diversity influences worker nutritional status. Apidologie 2015, 46(2), 150–63. [Google Scholar] [CrossRef]
- Büchler, R.; Costa, C.; Hatjina, F.; Andonov, S.; Meixner, M.D.; Conte, Y.L.; et al. The influence of genetic origin and its interaction with environmental effects on the survival of Apis mellifera L. colonies in Europe. J. Apic. Res. 2014, 53(2), 205–14. [Google Scholar] [CrossRef]
- Meixner, M.D.; Büchler, R.; Costa, C.; Francis, R.M.; Hatjina, F.; Kryger, P.; et al. Honey bee genotypes and the environment. J. Apic. Res. 2014, 53(2), 183–7. [Google Scholar] [CrossRef]
- Meixner, M.D.; Kryger, P.; Costa, C. Effects of genotype, environment, and their interactions on honey bee health in Europe. Curr. Opin. Insect Sci. 2015, 10, 177–84. [Google Scholar] [CrossRef]
- Bozina, K. How long does the queen live. Pchelovodstvo 1961, 38(6), 13. [Google Scholar]
- Seeley, T.D. Life history strategy of the honey bee, Apis mellifera. Oecologia 1978, 32(1), 109–18. [Google Scholar] [CrossRef]
- Page, R.E.; Peng, C.Y.S. Aging and development in social insects with emphasis on the honey bee, Apis mellifera L. Exp. Gerontol. 2001, 36(4-6), 695–711. [Google Scholar] [CrossRef]
- Jean-Prost, P.; Médori, P. Apiculture: know the bee, manage the apiary; Intercept Limited, 1994. [Google Scholar]
- Neupane, K.R.; Thapa, R.B. Pollen Collection and Brood Production by Honeybees (Apis mellifera L.) under Chitwan Condition of Nepal. J. Inst. Agric. Anim. Sci. 2005, 26(0), 143–8. [Google Scholar] [CrossRef]
- DeGrandi-Hoffman, G.; Gage, S.L.; Corby-Harris, V.; Carroll, M.; Chambers, M.; Graham, H.; et al. Connecting the nutrient composition of seasonal pollens with changing nutritional needs of honey bee (Apis mellifera L.) colonies. J. Insect Physiol. 2018, 109, 114–24. [Google Scholar] [CrossRef]
- Ulgezen, Z.N.; van Dooremalen, C.; van Langevelde, F. Why does resource availability matter for honeybee colonies in spring? Insectes Sociaux 2025, 72(4), 405–11. [Google Scholar] [CrossRef]
- Rueppell, O.; Bachelier, C.; Fondrk, M.K.; Page, R.E. Regulation of life history determines lifespan of worker honey bees (Apis mellifera L.). Exp. Gerontol. 2007, 42(10), 1020–32. [Google Scholar] [CrossRef]
- Requier, F.; Odoux, J.-F.; Henry, M.; Bretagnolle, V. The carry-over effects of pollen shortage decrease the survival of honeybee colonies in farmlands. J. Appl. Ecol. 2017, 54(4), 1161–70. [Google Scholar] [CrossRef]
- Pankiw, T.; Page, R.E. Genotype and colony environment affect honeybee (Apis mellifera L.) development and foraging behavior. Behav. Ecol. Sociobiol. 2001, 51(1), 87–94. [Google Scholar] [CrossRef]
- Wood, T.J.; Kaplan, I.; Szendrei, Z. Wild Bee Pollen Diets Reveal Patterns of Seasonal Foraging Resources for Honey Bees. Front. Ecol. Evol. 2018, 6(210). [Google Scholar] [CrossRef]
- Kandel, M.; E. El-Ansary, R.; B.M. Gomaa, M.; M. A. Abdel-Hameed, K.; F.M. Zaitoun, A. Evaluation of Hygienic Behaviour in Different Status of Managed Honey Bee Colonies. Alex. Sci. Exch. J. 2024, 45(3), 11–20. [Google Scholar] [CrossRef]
- Becher, M.A.; Osborne, J.L.; Thorbek, P.; Kennedy, P.J.; Grimm, V. REVIEW: Towards a systems approach for understanding honeybee decline: a stocktaking and synthesis of existing models. J. Appl. Ecol. 2013, 50(4), 868–80. [Google Scholar] [CrossRef]
- Walton, A.; Toth, A.L.; Dolezal, A.G. Developmental environment shapes honeybee worker response to virus infection. Sci. Rep. 2021, 11(1), 13961. [Google Scholar] [CrossRef]
- Knoll, S.; Pnna, W.; Varcasia, A.; Scala, A.; Cappai, M.G. The honey bee (Apis mellifera L., 1758) and the seasonal adaptation of productions. Highlights on summer to winter transition and back to summer metabolic activity. A review. Livest. Sci. 2020, 235, 104011. [Google Scholar] [CrossRef]
- Page, R.E.; Fondrk, M.K. The effects of colony-level selection on the social organization of honey bee (Apis mellifera L.) colonies: colony-level components of pollen hoarding. Behav. Ecol. Sociobiol. 1995, 36(2), 135–44. [Google Scholar] [CrossRef]
- Adam, B. Breeding the Honeybee: A contribution to the science of Beebreeding. In Scout Bottom Farm; Northern Bee Books: Mytholmroyd, Hebden Bridge, West Yorkshire, 1982; p. 118 p. [Google Scholar]
- Spivak, M.; Reuter, G.S. Performance of hygienic honey bee colonies in a commercial apiary. 1998. [Google Scholar] [CrossRef]
- Evans, J.D.; Aronstein, K.; Chen, Y.P.; Hetru, C.; Imler, J.L.; Jiang, H.; et al. Immune pathways and defence mechanisms in honey bees Apis mellifera. Insect Mol. Biol. 2006, 15(5), 645–56. [Google Scholar] [CrossRef]
- Büchler, R.; Andonov, S.; Bienefeld, K.; Costa, C.; Hatjina, F.; Kezic, N.; et al. Standard methods for rearing and selection ofApis mellifera queens. J. Apic. Res. 2013, 52(1), 1–30. [Google Scholar] [CrossRef]
- Uzunov, A.; Costa, C.; Panasiuk, B.; Meixner, M.; Kryger, P.; Hatjina, F.; et al. Swarming, defensive and hygienic behaviour in honey bee colonies of different genetic origin in a pan-European experiment. J. Apic. Res. 2014, 53(2), 248–60. [Google Scholar] [CrossRef]
- Brascamp, E.W.; Bijma, P. Methods to estimate breeding values in honey bees. Genet. Sel. Evol. 2014, 46(1), 53. [Google Scholar] [CrossRef]
- Uzunov, A.; Büchler, R.; Bienefeld, K. Performance testing protocol. A Guide for European Honey Bee Breeders. 2015. [Google Scholar]
- Uzunov, A.; Brascamp, E.W.; Du, M.; Bijma, P.; Büchler, R. Breeding Values in Honey Bees. Bee World 2023, 1–6. [Google Scholar] [CrossRef]
- Colin, T.; Bruce, J.; Meikle, W.G.; Barron, A.B. The development of honey bee colonies assessed using a new semi-automated brood counting method: CombCount. PLoS ONE 2018, 13(10), e0205816. [Google Scholar] [CrossRef]
- Capela, N.; Dupont, Y.L.; Rortais, A.; Sarmento, A.; Papanikolaou, A.; Topping, C.J.; et al. High accuracy monitoring of honey bee colony development by a quantitative method. J. Apic. Res. 2022, 1–10. [Google Scholar] [CrossRef]
- Delaplane, Keith S; Steen Jvd; Guzman-Novoa, E. Standard methods for estimating strength. [CrossRef]
- parameters of Apis mellifera colonies. J. Apic. Res. 2013, 52(1), 1–12. [CrossRef]
- Dainat, B.; Dietemann, V.; Imdorf, A.; Charriere, J.D. A scientific note on the ’Liebefeld Method’ to estimate honey bee colony strength: its history, use, and translation. Apidologie 2020, 51(3), 422–7. [Google Scholar] [CrossRef]
- Lazarov, S.; Dineva, G. An innovative method for determining the area of the capped brood in bee colonies. 2022. [Google Scholar]
- Meikle, W.G.; Holst, N. Application of continuous monitoring of honeybee colonies. Apidologie 2015, 46(1), 10–22. [Google Scholar] [CrossRef]
- Marchal, P.; Buatois, A.; Kraus, S.; Klein, S.; Gomez-Moracho, T.; Lihoreau, M. Automated monitoring of bee behaviour using connected hives: Towards a computational apidology. Apidologie 2020, 51(3), 356–68. [Google Scholar] [CrossRef]
- Vaudo, A.D.; Tooker, J.F.; Grozinger, C.M.; Patch, H.M. Bee nutrition and floral resource restoration. Curr. Opin. Insect Sci. 2015, 10, 133–41. [Google Scholar] [CrossRef]
- Page, R.E.; Laidlaw, H.H. Closed Population Honeybee Breeding. Bee World 1985, 66(2), 63–72. [Google Scholar] [CrossRef]
- Laidlaw, H.H.; Page, R.E. Queen rearing and bee breeding; Wicwas Press, 1997; p. 224 p. p. [Google Scholar]
- Moritz, R.F.A. Comparison of within-Family and Mass Selection in Honeybee Populations. J. Apic. Res. 1986, 25(3), 146–53. [Google Scholar] [CrossRef]
- Seeley, T.D. The lives of bees: the untold story of the honey bee in the wild; Princeton University Press, 2019. [Google Scholar]
- Bienefeld, K.; Ehrhardt, K.; Reinhardt, F. Genetic evaluation in the honey bee considering queen and worker effects - A BLUP-animal model approach. Apidologie 2007, 38(1), 77–85. [Google Scholar] [CrossRef]
- Büchler, R.; Berg, S.; Le Conte, Y. Breeding for resistance to Varroa destructor in Europe. Apidologie 2010, 41(3), 393–408. [Google Scholar] [CrossRef]
- Maucourt, S.; Fortin, F.; Robert, C.; Giovenazzo, P. Genetic Progress Achieved during 10 Years of Selective Breeding for Honeybee Traits of Interest to the Beekeeping Industry. Agriculture 2021, 11(6), 535. [Google Scholar] [CrossRef]
- Omholt, S.W.; Ådnøy, T. Effects of various breeding strategies on diploid drone frequency and quantitative traits in a honey bee population. Theor. Appl. Genet. 1994, 89(6), 687–92. [Google Scholar] [CrossRef]
- Kistler, T.; Basso, B.; Phocas, F. A simulation study of a honeybee breeding scheme accounting for polyandry, direct and maternal effects on colony performance. Genet. Sel. Evol. 2021, 53(1), 71. [Google Scholar] [CrossRef]
- Fürst, M.; McMahon, D.P.; Osborne, J.; Paxton, R.; Brown, M. Disease associations between honeybees and bumblebees as a threat to wild pollinators. Nature 2014, 506(7488), 364–6. [Google Scholar] [CrossRef]
- Seeley, T. Darwinian beekeeping: An evolutionary approach to apiculture. Am. Bee J. 2017, 157(3), 277–82. [Google Scholar]
- Robinson, G. Darwinian bee-keeping: lessons from the wild. Nature 2019, 571(7763), 34–6. [Google Scholar] [CrossRef]
- Neumann, P.; Blacquière, T. The Darwin cure for apiculture? Natural selection and managed honeybee health. Evol. Appl. 2017, 10(3), 226–30. [Google Scholar] [CrossRef]
- Neumann, P.; Beaurepaire, A.; Bouga, M.; Brodschneider, R.; Carreck, N.L.; Dahle, B.; et al. Darwin’s solution: Honeybees survive mite vectors and viruses through natural selection. Trends Parasitol. 2026. [Google Scholar] [CrossRef]
- Blacquière, T.; Boot, W.; Calis, J.; Moro, A.; Neumann, P.; Panziera, D. Darwinian black box selection for resistance to settled invasive Varroa destructor parasites in honey bees. Biol. Invasions 2019, 21(8), 2519–28. [Google Scholar] [CrossRef]
- Stearns, S.C. Trade-offs in life-history evolution. Funct. Ecol. 1989, 3(3), 259–68. [Google Scholar] [CrossRef]
- Roff, D.A. Life history evolution. 2002. [Google Scholar] [CrossRef]
- Zera, A.J.; Harshman, L.G. The physiology of life history trade-offs in animals. Annu. Rev. Ecol. Syst. 2001, 32(1), 95–126. [Google Scholar] [CrossRef]
- Li, S.; Yu, X.; Feng, Q. Fat body biology in the last decade. Annu. Rev. Entomol. 2019, 64(1), 315–33. [Google Scholar] [CrossRef]
- Arrese, E.L.; Soulages, J.L. Insect fat body: energy, metabolism, and regulation. Annu. Rev. Entomol. 2010, 55(1), 207–25. [Google Scholar] [CrossRef]
- Robert, E.; Page, J.; Metcalf, R.A. A Population Investment Sex Ratio for the Honey Bee (Apis mellifera L.). Am. Nat. 1984, 124(5), 680–702. [Google Scholar] [CrossRef]
- De la Rúa, P.; Jaffé, R.; Dall’Olio, R.; Muñoz, I.; Serrano, J. Biodiversity, conservation and current threats to European honeybees. Apidologie 2009, 40(3), 263–84. [Google Scholar] [CrossRef]
- Seeley, T.D. Honey bees of the Arnot Forest: a population of feral colonies persisting with Varroa destructor in the northeastern United States. Apidologie 2007, 38(1), 19–29. [Google Scholar] [CrossRef]
- Seeley, T.D.; Tarpy, D.R.; Griffin, S.R.; Carcione, A.; Delaney, D.A. A survivor population of wild colonies of European honeybees in the northeastern United States: investigating its genetic structure. Apidologie 2015, 46(5), 654–66. [Google Scholar] [CrossRef]
- Fries, I.; Imdorf, A.; Rosenkranz, P. Survival of mite infested (Varroa destructor) honey bee (Apis mellifera) colonies in a Nordic climate. Apidologie 2006, 37(5), 564–70. [Google Scholar] [CrossRef]
- Locke, B.; Fries, I. Characteristics of honey bee colonies (Apis mellifera) in Sweden surviving Varroa destructor infestation. Apidologie 2011, 42(4), 533–42. [Google Scholar] [CrossRef]
- Locke, B.; Conte, Y.L.; Crauser, D.; Fries, I. Host adaptations reduce the reproductive success of Varroa destructor in two distinct European honey bee populations. Ecol. Evol. 2012, 2(6), 1144–50. [Google Scholar] [CrossRef]
- Le Conte, Y.; de Vaublanc, G.; Crauser, D.; Jeanne, F.; Rousselle, J.-C.; Bécard, J.-M. Honey bee colonies that have survived Varroa destructor. Apidologie 2007, 38(6), 566–72. [Google Scholar] [CrossRef]
- Oddie, M.A.Y.; Dahle, B.; Neumann, P. Norwegian honey bees surviving Varroa destructor mite infestations by means of natural selection. PeerJ. 2017, 5, e3956. [Google Scholar] [CrossRef]
- Strauss, U.; Dietemann, V.; Human, H.; Crewe, R.M.; Pirk, C.W. Resistance rather than tolerance explains survival of savannah honeybees (Apis mellifera scutellata) to infestation by the parasitic mite Varroa destructor. Parasitology 2016, 143(3), 374–87. [Google Scholar] [CrossRef]
- Kefuss, J.; Vanpoucke, J.; Bolt, M.; Kefuss, C. Selection for resistance to Varroa destructor under commercial beekeeping conditions. J. Apic. Res. 2015, 54(5), 563–76. [Google Scholar] [CrossRef]
- Seeley, T.D. Life-history traits of wild honey bee colonies living in forests around Ithaca, NY, USA. Apidologie 2017, 48(6), 743–54. [Google Scholar] [CrossRef]
- Kefuss, J.; Vanpoucke, J.; De Lahitte, J.D.; Ritter, W. Varroa tolerance in France of intermissa bees from Tunisia and their naturally mated descendants: 1993-2004. Am. Bee J. 2004, 144(7), 563–8. [Google Scholar]
- Locke, B. Natural Varroa mite-surviving Apis mellifera honeybee populations. Apidologie 2016, 47(3), 467–82. [Google Scholar] [CrossRef]
- Locke, B.; Thaduri, S.; Stephan, J.G.; Low, M.; Blacquière, T.; Dahle, B.; et al. Adapted tolerance to virus infections in four geographically distinct Varroa destructor-resistant honeybee populations. Sci. Rep. 2021, 11(1), 12359. [Google Scholar] [CrossRef]
- Sokolov, N.A.; Boots, M.; Bartlett, L.J. Avoiding the tragedies of parasite tolerance in Darwinian beekeeping. Proc. R. Soc. B Biol. Sci. 2025, 292. [Google Scholar] [CrossRef]
- Jensen, A.B.; Palmer, K.A.; Boomsma, J.J.; Pedersen, B.V. Varying degrees of Apis mellifera ligustica introgression in protected populations of the black honeybee, Apis mellifera mellifera, in northwest Europe. Mol. Ecol. 2005, 14(1), 93–106. [Google Scholar] [CrossRef]
- Oleksa, A.; Chybicki, I.; Tofilski, A.; Burczyk, J. Nuclear and mitochondrial patterns of introgression into native dark bees (Apis mellifera mellifera) in Poland. J. Apic. Res. 2011, 50(2), 116–29. [Google Scholar] [CrossRef]
- Muñoz, I.; Henriques, D.; Johnston, J.S.; Chávez-Galarza, J.; Kryger, P.; Pinto, M.A. Reduced SNP Panels for Genetic Identification and Introgression Analysis in the Dark Honey Bee (Apis mellifera mellifera). PLoS ONE 2015, 10(4), e0124365. [Google Scholar] [CrossRef]
- Munoz, I.; De la Rua, P. Wide genetic diversity in Old World honey bees threaten by introgression. Apidologie 2021, 52(1), 200–17. [Google Scholar] [CrossRef]
- Bouga, M.; Alaux, C.; Bienkowska, M.; Büchler, R.; Carreck, N.L.; Cauia, E.; et al. A review of methods for discrimination of honey bee populations as applied to European beekeeping. J. Apic. Res. 2011, 50(1), 51–84. [Google Scholar] [CrossRef]
- Wallberg, A.; Han, F.; Wellhagen, G.; Dahle, B.; Kawata, M.; Haddad, N.; et al. A worldwide survey of genome sequence variation provides insight into the evolutionary history of the honeybee Apis mellifera. Nat. Genet. 2014, 46(10), 1081–8. [Google Scholar] [CrossRef]
- Wragg, D.; Eynard, S.E.; Basso, B.; Canale-Tabet, K.; Labarthe, E.; Bouchez, O.; et al. Complex population structure and haplotype patterns in the Western European honey bee from sequencing a large panel of haploid drones. Mol. Ecol. Resour. 2022, 22(8), 3068–86. [Google Scholar] [CrossRef]
- Chen, C.; Parejo, M.; Momeni, J.; Langa, J.; Nielsen, R.O.; Shi, W.; et al. Population Structure and Diversity in European Honey Bees (Apis mellifera L.)—An Empirical Comparison of Pool and Individual Whole-Genome Sequencing. Genes. 2022, 13(2), 182. [Google Scholar] [CrossRef]
- Parejo, M.; Kryger, P.; Bouga, M.; Dall’Olio, R.; Kandemir, I.; Costa, C. Conserving Locally Adapted Honey Bees. In Sustainable Honey Bee Breeding: A Scientific Guide for Future Beekeeping; Springer, 2025; pp. 53–65. [Google Scholar]
- Ruttner, F. Methods of Breeding Honeybees: Intra-Racial Selection or Inter-Racial Hybrids? Bee World 1968, 49(2), 66–72. [Google Scholar] [CrossRef]
Figure 1.
Drones laid by the queen. The spermatozoa of one drone are haploid and genetically identical.
Figure 1.
Drones laid by the queen. The spermatozoa of one drone are haploid and genetically identical.
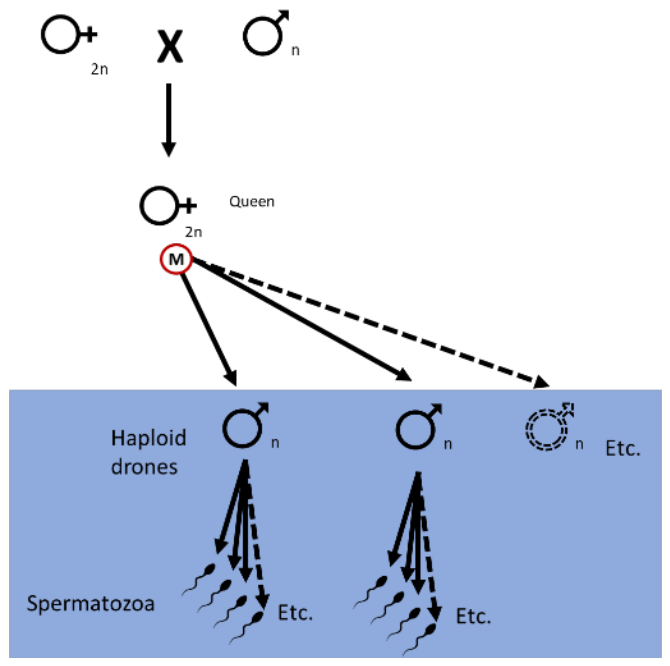
Figure 2.
Drones-laying workers increase genetic diversity of drones.
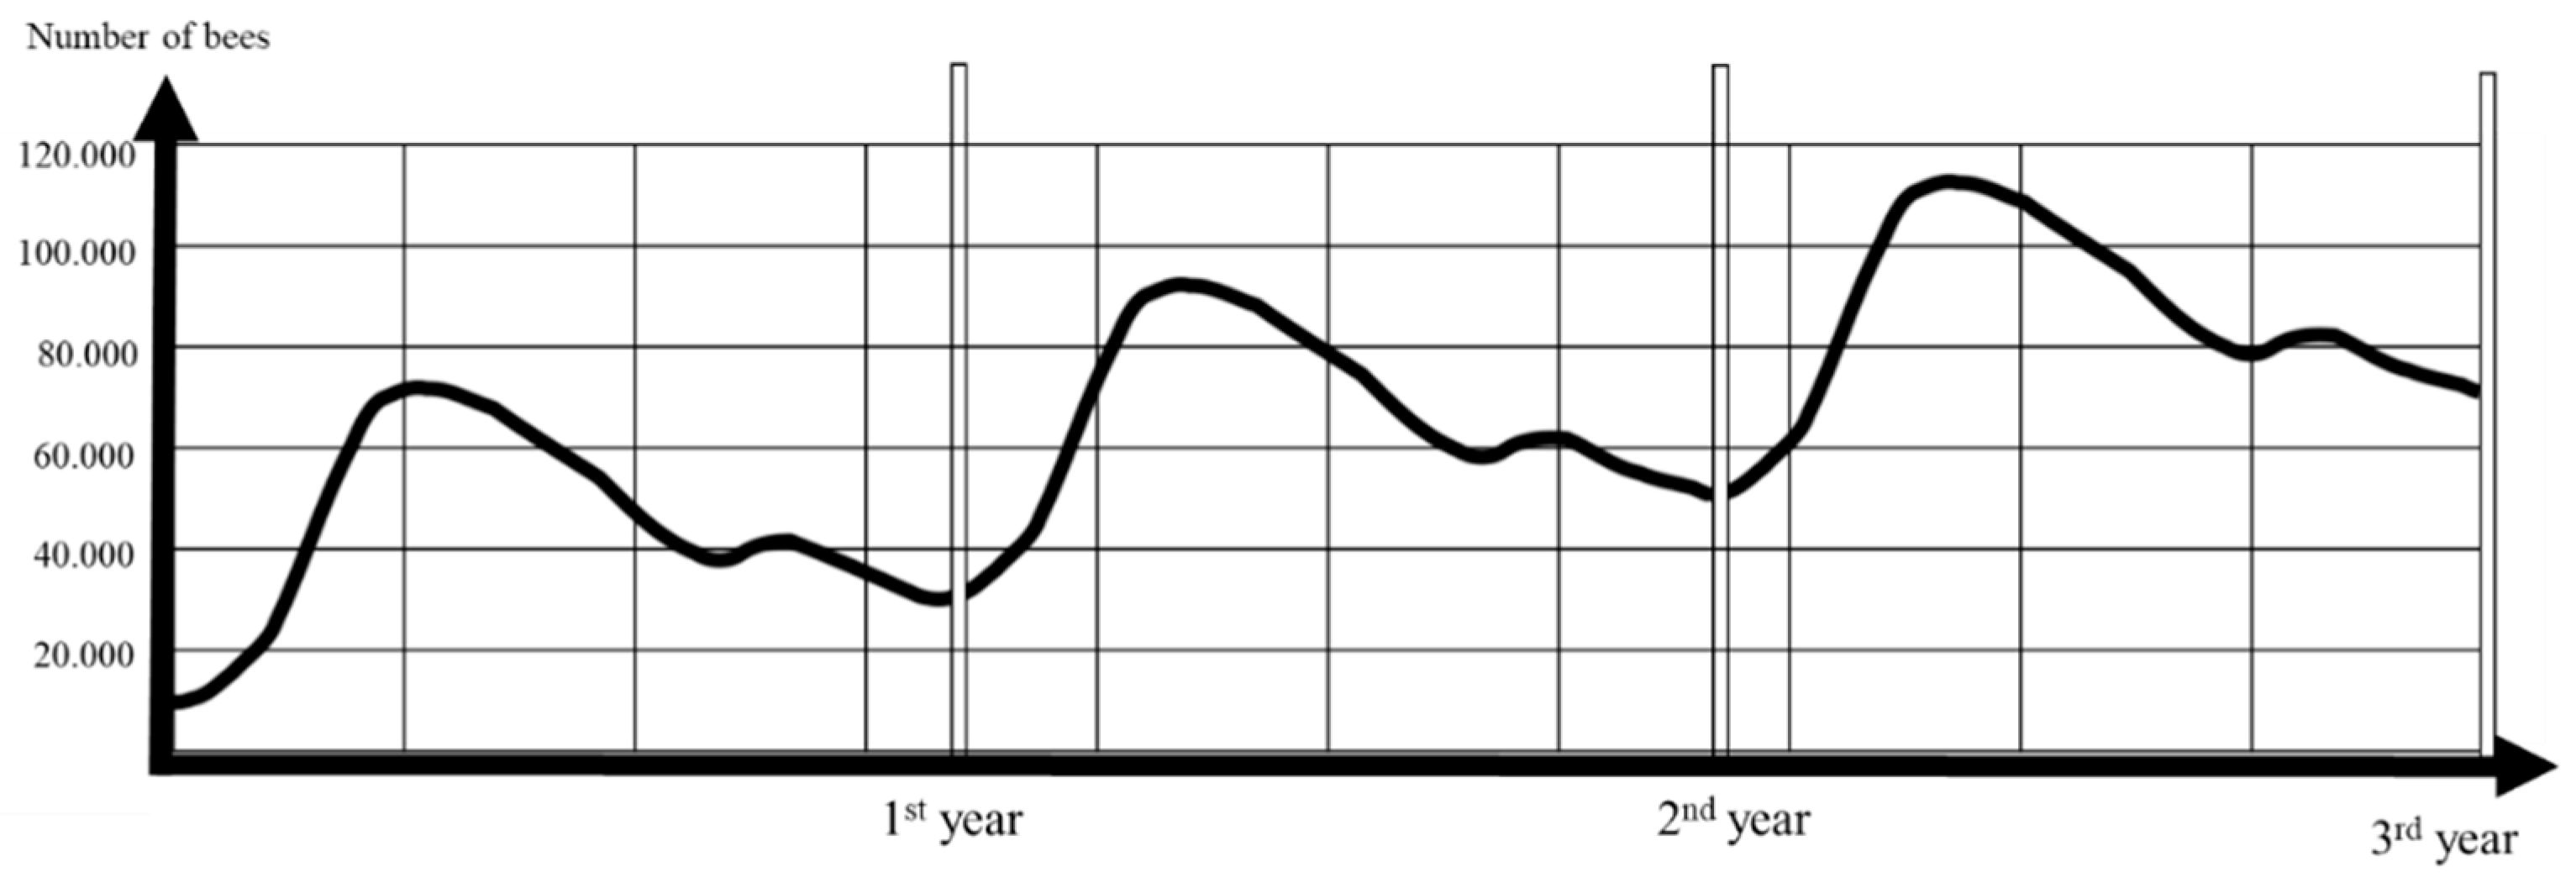
Figure 3.
Multiple mating of a virgin queen.
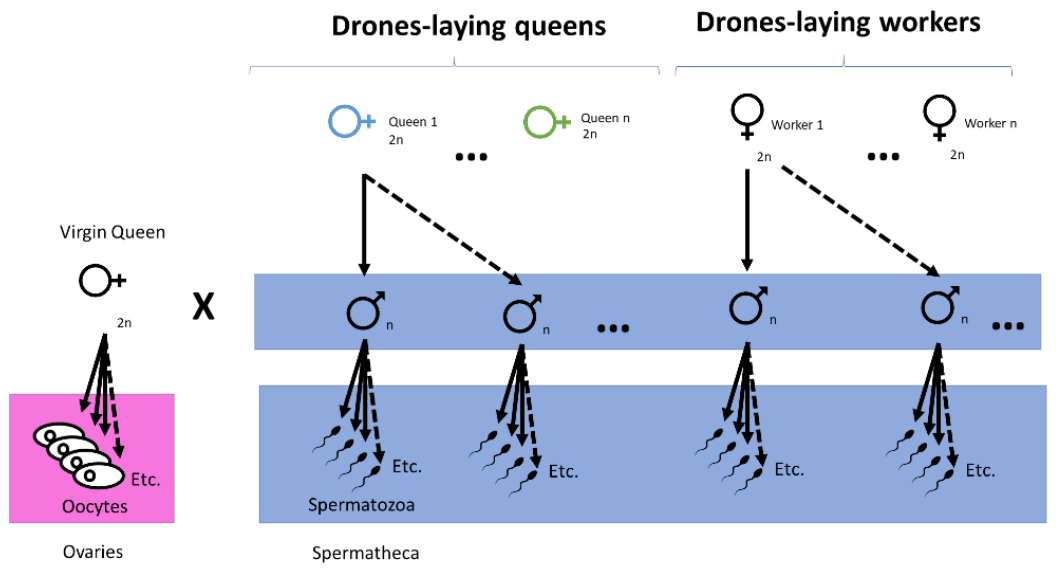
Figure 4.
Genetic architecture of the honeybee colony.
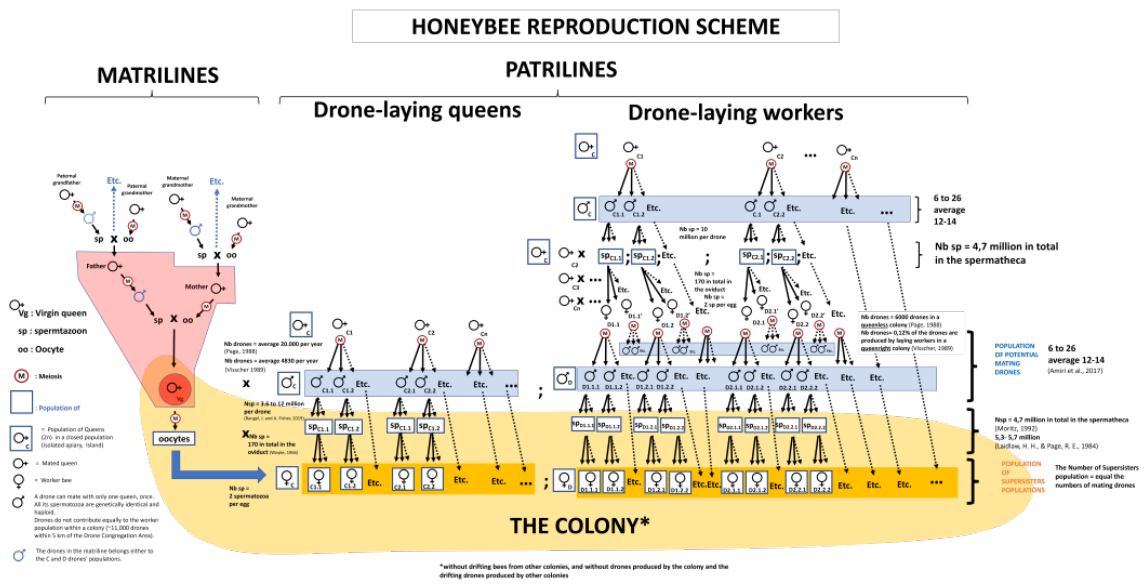
Figure 6.
An integrated conservation–breeding framework.
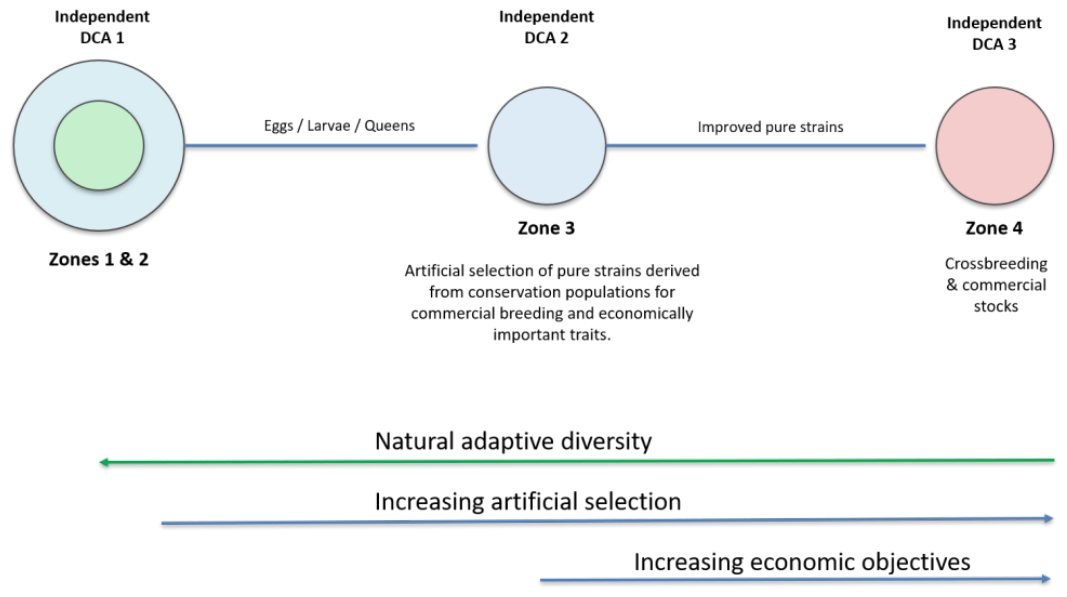
Figure 7.
Example of a controlled inter-racial hybrid breeding scheme.
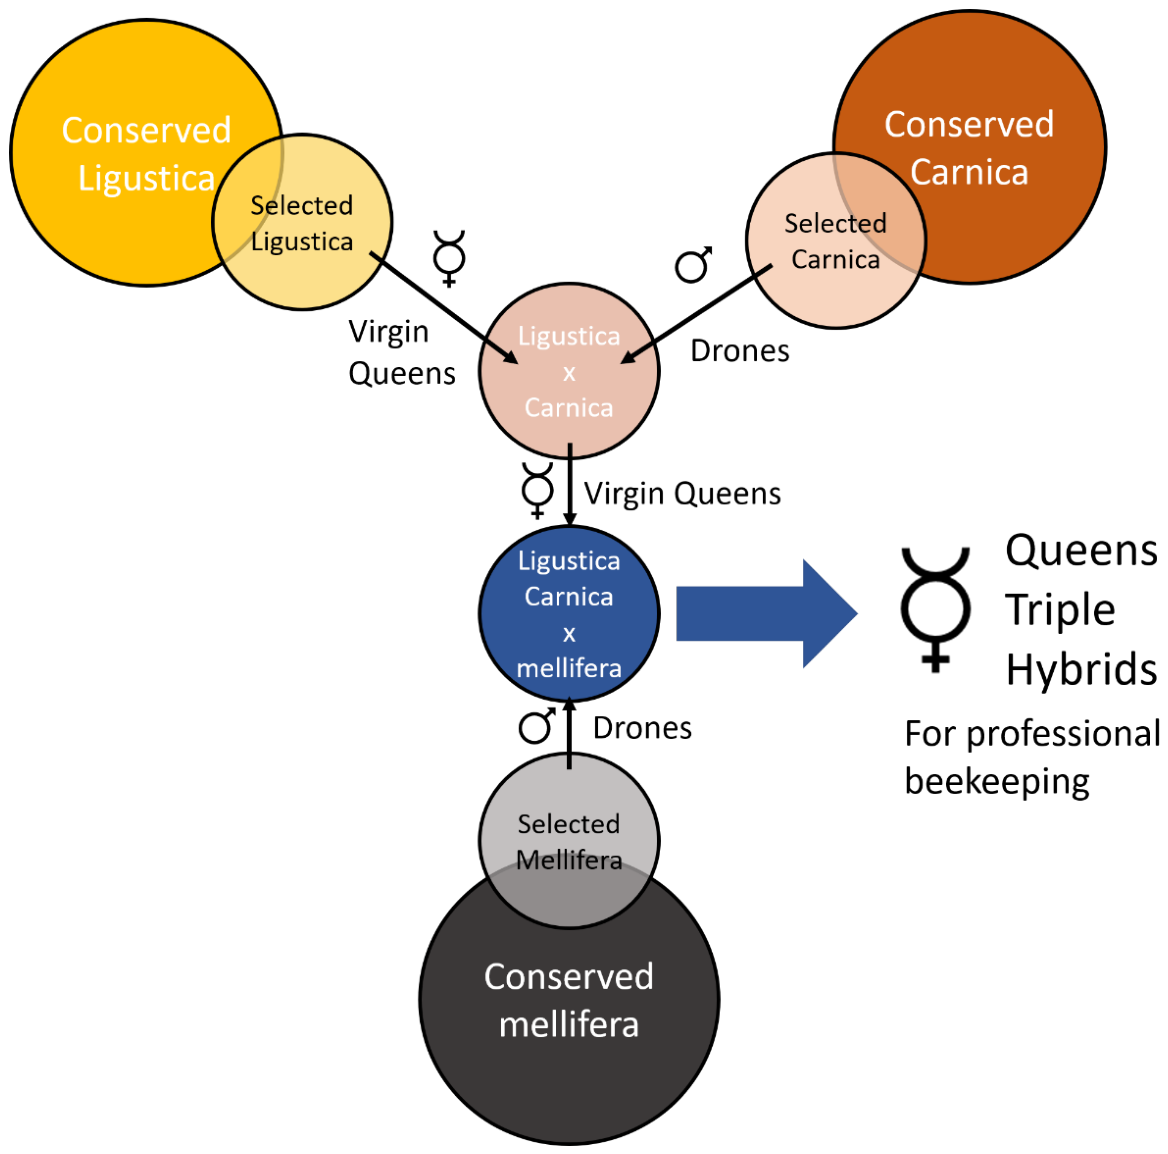

Table 1.
Chronological review of estimates of the number of drones mating with the queen.
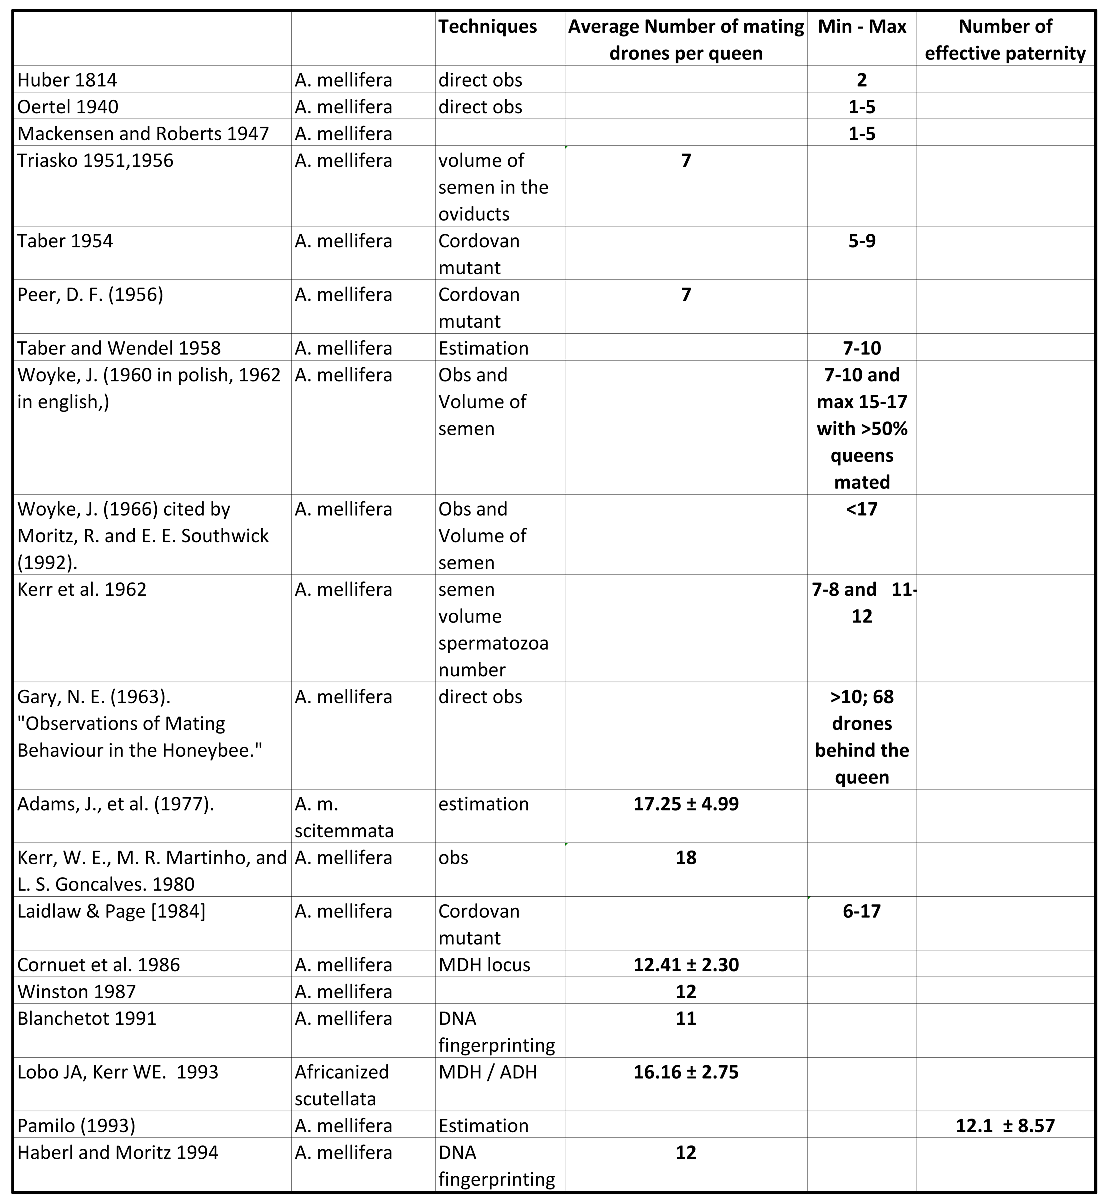
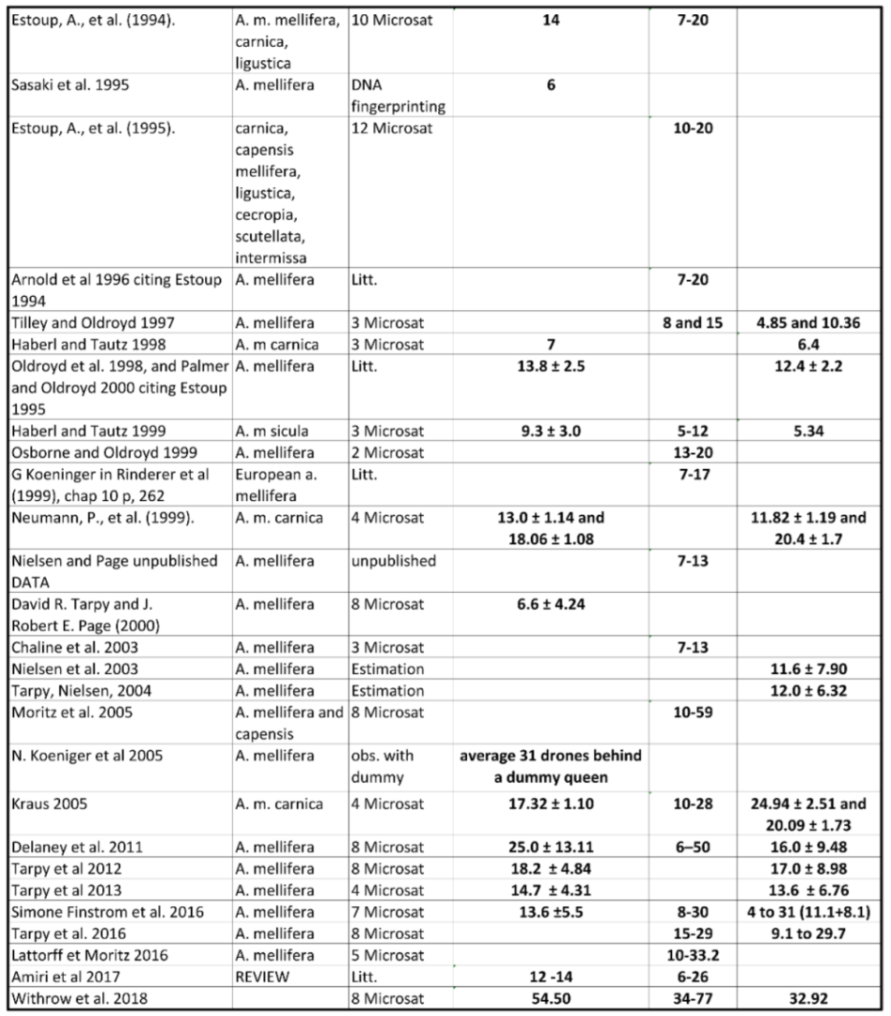
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (http://creativecommons.org/licenses/by/4.0/).
Copyright: This open access article is published under a Creative Commons CC BY 4.0 license, which permit the free download, distribution, and reuse, provided that the author and preprint are cited in any reuse.