
Submitted:
08 September 2026
Posted:
16 September 2026
You are already at the latest version
Abstract
Foot-and-mouth-disease is a highly contagious disease affecting cloven hoofed animals, having an important direct and indirect socio-economic impact in livestock industry. The disease has been successfully eradicated from some regions, but it is still endemic in most of the world. The use of vaccines that contain strains that match antigenically with the FMD strains circulating in the field is one of the main tools, together with a good epidemiology plan for its eradication. Supplying information in relation to characterization of circulating strains is useful to maintain antigen banks updated in order to be prepared to attend eventual incursions. Previously, information has been published in relation to genetic changes in the evolution of type O circulating lineages in Vietnam and other countries of Southeast Asia. Here we present genetic and antigenic characterization of type O viral strains circulating in Vietnam during 2019 until 2024, vaccine matching tests were performed using a swine sera pool collected from animals vaccinated with a monovalent vaccine containing O1 Campos strain at 28 days-post-vaccination (dpv). High neutralizing antibody titers were registered for type O isolates with r1 values over 0.3 in most of the cases, indicating good cross-reactivity. Furthermore, a swine challenge test performed against one of field isolates from the Mya-98 lineage exhibited 100% protection even with a single vaccine dose. All together these results demonstrate that high potency O1 Campos vaccines could be used for controlling outbreaks in endemic regions with circulation of multiple type O topotypes and lineages.
Keywords:
FMD in vivo challenge vaccine coverage
; SEA Mya98 cross protection study
; FMDV circulation in Vietnam
Introduction
Foot-and-mouth-disease (FMD) is a highly contagious disease affecting cloven-hoofed animals and has significant socio-economic impact on the livestock industry due to restriction of animal movements and trade, as well as severe production losses. FMD virus is a member of the family Picornaviridae, genus Aphtovirus [1]. VP1 sequence analysis is widely used for the genetic characterization of Foot and Mouth Disease Virus (FMDV) and for the classification of viruses into topotypes and lineages. Foot-and-mouth disease virus is classified into seven antigenically distinct serotypes, and serotype O is further divided into 11 topotypes [2,3]. Livestock plays a crucial role in Vietnam's agricultural sector, contributing to both food security and the national economy. The raising of cattle, pigs, sheep and poultry is essential for food production in the country, with pork and chicken being especially popular in the local diet. According to the WHOA, the Republic of Vietnam currently has an endemic status of Foot-and-mouth-disease. Previous reports have been published in relation to genetic and antigenic characterization of circulating strains in the region [4,5,6].
Having updated information available in essential for analyzing and making informed decisions regarding the potential updating of antigen banks, emergency vaccine banks, or epidemiological strategies to fight the disease. The present work provides an updated analysis, focusing on serotype O isolates that have been circulating in the last years [7,8,9] reporting the genetic and antigenic characterization of 33 viral isolates collected from outbreaks between 2019 and 2024 in Vietnam. The genetic analysis revealed a relevant genetic change for the mya-98 lineage that correlates with other reports [10,11] and informal communications received from veterinary officers in different countries of Southeast Asia at the WOAH reference laboratory at SENASA, Argentina. The O1 Campos monovalent vaccine used in this study for antigenic characterization demonstrated a robust potency with high cross-reactivity against most Vietnamese local field strains. An in vivo trial also correlated with the in vitro results obtaining 100% of efficacy.
Materials and Methods
Samples collection and viral isolation and amplification: A total of 33 FMDV positive serotype O samples collected in Vietnam by the Regional Animal Health Office No. 6 (RAHO 6), the Department of Animal Health, and the National Centre for Veterinary Diagnosis were submitted to the FMD Reference Laboratory at SENASA, Argentina, for molecular characterization and further analysis.
Epithelial tissue samples collected in the field were processed by grinding amplified in the cell line BHK-21 (baby hamster kidney) clone 13 under the same conditions as stated before [6]. The whole process was carried out in containment facilities, according to the standards of the World Organization for Animal Health (WOAH) of the National Agro-food Health and Quality Service (SENASA) of Argentina. Virus amplification was carried out by infecting confluent monolayers (80%-100%) of BHK-21 cells. Each viral stock was titrated by the end-point dilution method,
Genetic characterization: Nucleotide sequencing: Procedures for RNA extraction, amplification and sequencing conditions applied to determine the complete VP1 coding sequence of the viral isolates were already published [5,12]. The nucleotide sequences were determined using the BigDye ® Terminator v3. 1 Cycle Sequencing Kit (Applied Biosystems), following the manufacturer’s procedure. The reaction product was purified by ethanol/EDTA precipitation; the recovered material was dyed. For Reading, the dyed samples were resuspended in formamide 10% as recommended for use in a 3500 Genetic Analyzer machine (Aplied Biosystems).
Sequence and Phylogenetic analysis: VP1 nucleotide and amino acid sequences were edited and aligned using Bioedit software v7.2.5. Pairwise sequence identity matrices were generated in MEGA12 using p-distance method, and the same software was used for phylogenetic inference [13]. The phylogenetic tree was constructed with MEGA12. The best-fitting evolutionary model was selected according to the Bayesian Information Criterion (BIC) and the corrected Akaike Information Criterion (AICc). The Tamura-Nei 1993 model with Gamma-distributed rate variation among sites and a proportion of invariant sited (TN93+G+I) was used. Phylogenetic relationships among FMDV serotype O strains were inferred from VP1 nucleotide sequences using the Maximum Likelihood method, and branch support was assessed with 1.000 bootstrap replicates. The final dataset comprised 101 coding nucleotide sequences and 633 positions.
Antigenic characterization, in vitro antigenic analysis of field isolates: Vaccine matching was assessed by a bidimensional virus neutralization test (VNT), followed by r1-value calculation, as previously described [6]. Pools of swine sera collected at 28 days post-vaccination (dpv) from animals immunized with a commercial monovalent oil-adjuvanted O1 Campos vaccine (Biogénesis Bagó S.A.) were used. The O1 Campos virus strain included in the in vitro assays was obtained from the virus collection of the FMD Reference Laboratory in Argentina.
In vivo challenge test: Animal experiments were conducted in accordance with the guidelines of the Institutional Committee for the Care and Use of Laboratory/Experimental Animals of SENASA, Argentina. The FMDV serotype O strain SEA Mya-98 O/VTN/24FS02/2024 was selected for the in vivo challenge experiment. Prior to the challenge, a single passage in pigs was performed to obtain the challenge virus stock. Briefly, two-month-old naïve Landrace x Large White pigs, obtained from a commercial farm, were inoculated with 100.000 TCID50/mL of virus. Epithelial tissue and vesicular fluid were collected at seventy-two hours post-inoculation, homogenized in cell culture medium at a 1:5 dilution, processed titrated and stored at -80°C until use. Vaccination and challenge were performed following the scheme recommended for cattle in the European Pharmacopoeia [14], adapted to pigs. Two groups of ten pigs were challenged. In group 1, pigs received a single full dose of a commercial monovalent O1 Campos vaccine 28 days before challenge. The vaccine was administered intramuscularly in the neck region at a volume of 2 mL. In group 2, pigs were vaccinated 56 days before challenge and revaccinated 28 days after the first vaccination. Two naïve pigs were included as unvaccinated controls for each group. Seventy-two hours before challenge, animals were transferred to WOAH biosafety level 4 animal facilities. Vaccinated animals and unvaccinated controls were housed in separate rooms with independent air-handling systems. Vaccinated groups were kept without direct contact between groups and were provided with separate feed and water troughs. For the challenge, pigs were inoculated intramuscularly with 100.000 infectious doses (ID) of the pig-adapted O/VTN/24FS02/2024 strain in a final volume of 1 mL. Animals were monitored daily for clinical signs of FMD for 7 days after challenge. Animals showing generalized lesions were considered non-protected, whereas animals without clinical generalization were considered protected. Serum samples were collected at different time points before and after vaccination, revaccination, and challenge. Antibody titers against the vaccine strain and the field isolate were determined by bidimensional virus neutralization test (VNT), as previously described [6].
Results
Genetic Characterization
In this study, sequence analysis of the 33 FMDV isolates revealed that all of them belong to viral serotype O. The nucleotide sequences of the complete VP1 coding region have been submitted to National Center Biotechnology Information (NCBI) (Accession No. Table 1).
The VP1 nucleotide sequences were then compared with 68 previously published FMDV sequences to assess their phylogenetic relationships. The results showed that the Vietnamese isolates clustered into three distinct lineages within two topotypes: ME-SA/PanAsia, ME-SA/Ind-2001, and SEA/Mya-98 (Figure 1).
Six isolates clustered within the ME-SA topotype, PanAsia lineage, showing 88,13-100% nucleotide identity and 94,79-100% amino acid identity among sequences conforming this lineage. Twenty-one isolates grouped into the ME-SA topotype, ind-2001 lineage, with 91,31-99,84% nucleotide identity and 96,21-100% amino acid identity within the lineage. The remaining six isolates clustered into the SEA topotype, Mya-98 lineage, showing 84,83-100% nucleotide and 88,63-100% amino acid identity, intra-lineage (data not shown).
Nucleotide and amino acid identities between the Vietnamese isolates and the vaccine strain O1 Campos (Accession n. AJ320488) were also evaluated. Compared with O1 Campos, PanAsia isolates showed 77,07-78,66% nucleotide identity and 86,85-87,93% amino acid identity; Ind-2001 isolates showed 72,68-75,01% nucleotide identity and 86,31-87,39% amino acid identity; and Mya-98 isolates showed 70,66-74,53% nucleotide identity and 84,66-85,76% amino acid identity (supplementary, Table S1.).
Variation in the Amino Acids of the VP1 Gene
Amino acid differences between the FMDV isolates and FMDV reference strains for each lineage were analyzed within the main antigenic regions of VP1: BC-loop region (residues 40-60), GH-loop region (residues 130-160) and C-terminal region (residues 200-211) [15]. Interesting, for the Ind-2001 lineage, several substitutions were observed at position 45, 49, 59, 138-142, 153 and 155. Notably, substitutions at positions E138G, A140P and T142A in O/VTN/24FS55/2024 involve polar to non-polar changes. Regarding the Mya-98 lineage, amino acid changes were detected at positions 50, 135, 156 and 209. A V209T substitution implicating a polarity change, was observed in isolates O/VTN/24FS02/2024, O/VTN/24FS19/2024, O/VTN/24FS54/2024 and O/VTN/24FS56/2024. Within the PanAsia lineage, notable differences were also observed among the most recent isolates. O/VTN/24FS05/2024, O/VTN/24FS17/2024, O/VTN/24FS10/2024, O/VTN/24FS11/2024 and O/VTN/24FS15/2024 showed a P140S substitution, involving a change from non-polar to polar residue. In addition, O/VTN/24FS11/2024 showed a conservative R157K substitution. The RGD motif, located at amino acid positions 145–147, was fully conserved among all isolates and reference strains analyzed (data not shown). The alignments of VP1 amino acid sequences for each lineage are shown in supplementary figures 1-3.
When comparing main VP1 antigenic regions between the isolates reported in this work and the O1 Campos vaccine strain (Figure 2), for those belonging to the Ind-2001 lineage substitutions were found at position 45-46, 50, 56, 58-59, 133, 135, 137-142, 153, 155 and 156.; whereas PanAsia isolates present substitutions at positions 46, 50, 56, 58, 133, 137-140, 142 and 155-157; and Mya-98 isolates show differences at positions 45-48, 50, 56, 58, 133, 135, 137-141, 153, 155-156, 158 and 209.
Antigenic Analysis
Vaccine matching studies were performed using monovalent O1 Campos vaccine strain in order to assess the antigenic relationship of this vaccine strain with Vietnamese field isolates. The mean neutralization antibody titer against the homologous strain was 2.16 Log10 across the different sets of tests. Post-vaccination swine sera pool collected at 28 dpv showed satisfactory heterologous neutralizing titers (>1.5 Log10) against the tested isolates. Although most isolates showed r1 values above 0.3, three isolates, O/VTN/20-200/2020, O/VTN/24FS12/20245, and O/VTN/24FS56/2024, had r1 values below this threshold (Table 2). These findings suggest that O1 Campos has a good antigenic relationship with representative Vietnamese serotype O viruses from the Ind-2001, Mya-98 and PanAsia lineages.
In Vivo Challenge
To confirm the in vitro results for type O 2024 strains that showed a genetic divergence to vaccine strain, an in vivo challenge test with O/VTN/24FS02/2024 strain was performed as indicated in materials and methods. Control animals showed lesions in the four feet, tongue, nose and mouth cavity demonstrating viral generalization. In both groups of animals, those challenged at 28 DPV after a single vaccination (n = 10) and those challenged after receiving a booster dose at 28 days post vaccination (n = 10), showed 100% protection. Consequently, the vaccine conferred full protection against the heterologous challenge. Sera from the animals obtained at 0 dpv were negative for VNT antibodies detection. At the time of challenge test, mean heterologous VNT titers (Log10) were 1.58 for animals in group 1 (sd 0.07) and 2.40 for group 2 (sd 0.18). These values are consistent with in-vitro test described before.
Discussion
Identifying effective vaccines and vaccine strains to control FMD outbreaks that may spread to new regions is essential for preparedness and disease control. Continuous monitoring of vaccine strains included in strategic antigen reserves is therefore critical to ensure their suitability against contemporary field strains. In this context, the present study provides updated evidence on the antigenic and protective performance of the O1 Campos vaccine strain against FMDV serotype O isolates circulating in Vietnam up to 2024.
The O1 Campos vaccine strain has been widely and successfully used in South America and has also been included in vaccination strategies or vaccine banks for other regions, including parts of Asia [5,6,16,17]. Previous studies have shown that high-quality vaccines formulated with O1 Campos can induce protective immunity against heterologous serotype O strains belonging to different genetic lineages [5,6,16]. The present results further support this observation, since Vietnamese isolates belonging to three distinct lineages, SEA/Mya-98, ME-SA/Ind-2001 and ME-SA/PanAsia, showed evidence of antigenic relationship with O1 Campos.
Phylogenetic analysis confirmed that the 33 Vietnamese isolates analyzed in this study were distributed into three major lineages. Despite the genetic diversity observed among them, particularly between ME-SA and SEA topotypes, the in vitro and in vivo results suggest that a high-quality monovalent O1 Campos vaccine may provide relevant cross-protection against representative contemporary Vietnamese FMDV serotype O strains. This is particularly important for emergency vaccination scenarios, where rapid deployment of an available and well-characterized vaccine strain is required.
Analysis of VP1 amino acid sequences revealed several amino acid substitutions in antigenically relevant sites, particularly in the GH loop within Ind-2001, Mya-98 and PanAsia lineages. Although some substitutions may contribute to local conformational or antigenic variation, their functional impact should be interpreted in the context of serological and challenge data.
Most isolates showed r1 values consistent with a good antigenic relationship with the O1 Campos vaccine strain. However, three isolates, O/VTN/20-200/2020, O/VTN/24FS12/2024 and O/VTN/24FS56/2024, showed reduced in vitro vaccine matching values based on r1 determination. This finding highlights an important limitation of interpreting r1 values in isolation.
Although r1 values are widely used as an indicator of antigenic relationship between strains, the association with in-vivo protection may vary depending on the overall formulation, including antigen payload, adjuvant composition, manufacturing quality, and appropriate dosing intervals. It has been observed that high potency vaccines can confer protection even when reduced cross-reactivity is observed in vitro [18,19].
For this reason, r1 values should be interpreted together with complementary serological and biological data. In the present study, VNT antibody titers obtained using sera from vaccinated animals provided additional evidence of expected protection. The analysis of pooled sera neutralizing antibody levels, revealed titer > 1.5 for all tested isolates, supporting the broad protective potential of the O1 Campos vaccine. A heterologous titer of 1.5 has been widely used recently as an indicator of likely cross-protection [20].
Moreover, the in vivo heterologous challenge performed with the O/VTN/24FS02/2024, which presented r1 value ranging from 0.25 to 0.46 in different determinations (mean value 0.33). This strain was selected for the challenge test due to its capacity to better replicate into cell culture conditions in relation to other isolates showing low r1 values. In vivo results confirmed the in vitro prediction based on the antibody titers (mean value 1.5 for animals with a single dose), as vaccinated and revaccinated animals were fully protected even with a single vaccine dose.
Overall, the results reinforce the value of integrating phylogenetic characterization, VP1 amino acid analysis, r1-value determination, VNT antibody titers and in vivo challenge studies when assessing vaccine suitability. The findings support the continued relevance of the O1 Campos vaccine strain as a candidate for protection against diverse FMDV serotype O lineages circulating in Vietnam [21,22]. However, the genetic and antigenic variability observed among contemporary isolates underscores the need for continued surveillance of circulating strains and periodic reassessment of vaccine matching.
Conclusions
Evidence of the suitability of including O1 Campos Strain in high-quality vaccines for conferring cross-reactivity and protection against recent Vietnamese circulating strains has been provided.
These findings are consistent with previous results supporting that the use of a high-potency, good-quality vaccine elicits a cross-reactive immune response. In this sense, a vaccine strain belonging to the EURO-SA topotype showed high antibody titers against all Vietnamese isolates belonging to SEA/Mya 98, CATHAY and ME-SA/PanAsia [6].
Re-emerging strains indicate that the virus adapts through local evolution in pigs and cattle, highlighting the need of regular monitoring and updates of vaccine strains.
Author Contributions
DC: methodology, Data Curation, writing, revision, Software, images CM: methodology, bench work, writing, revision, Software, images VVH: methodology, review and edition NTP: methodology, review and edition AIT: methodology, Data Curation, Supervision SC: conceptualization, writing, editing and review CM: methodology SGN: conceptualization, Methodology, Data Curation, writing, editing and review, resources, Software, Supervision.
Funding
Laboratory work was funded with SENASA’s own resources. Sample collection and research in identification was funded by RAHO 6, DAH Vietnam and the National Centre for Veterinary Diagnosis, Vietnam.
Informed Consent Statement
Informed consent was obtained from all subjects involved in the study.
Data Availability Statement
All data is available upon request to the authors.
Conflicts of Interest
The author(s) declare(s) that there is no conflict of interest regarding the publication of this paper.
References
- Bachrach, H.L. “Foot-and-mouth disease”. Annu Rev. Microbiol. 1968, vol.22, 201–244. [Google Scholar]
- Samuel, A.R.; Knowles, N.J. “Foot-and-mouth disease type O viruses exhibit genetically and geographically distinct evolutionary lineages (topotypes)”. J. Gen. Virol. 2001, vol. 82, 609–621. [Google Scholar] [CrossRef]
- Kitching, R.P.; Knowles, N.J.; Samuel, A.R.; et al. “Development of foot and- mouth disease virus strain characterisation–a review”. Trop. Anim. Health Prod. 2001, Vol. 21(3), 153–66. [Google Scholar]
- Galdo Novo, S.; Malirat, V.; Maradei, E.D.; et al. “Antigenic and immunogenic spectrum of Foot-and- Mouth Disease vaccine strain O 1 Campos against representative viruses of topotypes that circulated in Asia over the past decade. 2017”. Vaccine 2017, Vol. 35, p1016. [Google Scholar] [CrossRef] [PubMed]
- Galdo Novo, S.; Malirat, V.; Maradei, E.D.; et al. “Efficacy of a high quality O1 Campos foot-and-mouth disease vaccine upon challenge with a heterologous Korean O Mya98 lineage virus in pigs. 2018”. Vaccine 2018, Vol. 36, 15. [Google Scholar] [CrossRef] [PubMed]
- Taffarel, A.I.; Barrios Benito, M.Y.; Hung, V.V.; Cardillo, S.; Phuong, N.T.; Caldevilla, C.; Galdo Novo, S. Foot-and-mouth disease virus strains isolated in Vietnam during 2010-2019: genetic characterization and antigenic relatedness to the Euro SA vaccine. Arch. Virol. 2024, 169(3), 44. [Google Scholar] [CrossRef] [PubMed]
- Le, V.P.; Nguyen, T.; Lee, K.N.; et al. “Molecular characterization of serotype A foot-and-mouth disease viruses circulating in Vietnam in 2009”. Vet. Microbiol. 2010, Vol. 144(1–2), 58–66. [Google Scholar] [CrossRef] [PubMed]
- Le, V.P.; Nguyen, T.; Park, J.H.; et al. “Heterogeneity and genetic variations of serotypes O and Asia 1 foot-and-mouth disease viruses isolated in Vietnam”. Vet. Microbiol. 2010, Vol. 145(3–4), 220–9. [Google Scholar] [CrossRef] [PubMed]
- Le, V.P.; Vu, T.T.H.; Duong, H.Q.; et al. “Evolutionary phylodynamics of foot-and-mouth disease virus serotypes O and A circulating in Vietnam”. BMC Vet. Res. 2016, Vol. 12, 269. [Google Scholar]
- Khanh, N.P.; Khang, T.D.; Lam, N.T.; Trang, C.T.H.; Hoang, L.T. Molecular Characterization and Genetic Diversity of Isolated Foot-and-Mouth Disease Viruses Circulating in Cattle in The Mekong Delta Provinces, Vietnam. Vet. Med. Int. 2025, 2025, 6680850. [Google Scholar] [CrossRef] [PubMed] [PubMed Central]
- Khang, T.D.; Khanh, N.P. Phylogenetic and genotypic characteristics of foot-and-mouth-disease virus in cattle in Tra Vinh province, Vietnam. Vet. World 2024, 17(12), 2858–2864. [Google Scholar] [CrossRef] [PubMed] [PubMed Central]
- Malirat, V.; Franca de Barros, J.J.; Bergmann, I.E.; et al. “Phylogenetic analysis of foot-and-mouth disease vírus type O re-remerging in free areas of South America”. Virus Res. 2007, vol.124, 22–8. [Google Scholar] [CrossRef] [PubMed]
- Kumar, S.; Stecher, G.; Suleski, M.; Sanderford, M.; Sharma, S.; Tamura, K. MEGA12: Molecular Evolutionary Genetic Analysis Version 12 for Adaptive and Green Computing. Mol. Biol. Evol. 2024, Volume 41(Issue 12), msae263. [Google Scholar] [CrossRef] [PubMed]
- European Pharmacopoeia. Foot-and-mouth disease (ruminants) vaccine (inactivated) Eur. Ph. In /2017, 0063, 9th ed.; 2017; Vol. 01. [Google Scholar]
- Asfor, A. S.; Upadhyaya, S.; Knowles, N. J.; King, D. P.; Paton, D. J.; Mahapatra, M. Novel antibody binding determinants on the capsid surface of serotype O foot-and-mouth disease virus. J. General. Virol. 2014, 95 Pt 5, 1104–1116. [Google Scholar] [CrossRef] [PubMed]
- Yang, M.; Xu, W.; Goolia, M.; Zhang, Z. Characterization of monoclonal antibodies against foot-and-mouth disease virus serotype O and application in identification of antigenic variation in relation to vaccine strain selection. Virol. J. 2014, 11, 136. [Google Scholar] [CrossRef] [PubMed]
- Harmsen, M. M.; Li, H.; Sun, S.; Van der Poel, W. H. M.; Dekker, A. Mapping of foot-and-mouth disease virus antigenic sites recognized by single-domain antibodies reveals different 146S particle specific sites and particle flexibility. Front. Vet. Sci. 2023, 9, 1040802. [Google Scholar] [CrossRef] [PubMed]
- Yang, F.; Zhu, Z.; Cao, W.; Liu, H.; Wei, T.; Zheng, M.; Zhang, K.; Jin, Y.; He, J.; Guo, J.; Liu, X.; Zheng, H. Genetic Determinants of Altered Virulence of Type O Foot-and-Mouth Disease Virus. J. Virol. 2020, 94(7), e01657-19. [Google Scholar] [CrossRef] [PubMed] [PubMed Central]
- Brehm, K.E.; Kumar, N.; Thulke, H.H.; Haas, B. High potency vaccines induce protection against heterologous challenge with foot-and-mouth disease virus. Vaccine 2008, 26(13), 1681–7. [Google Scholar] [CrossRef] [PubMed]
- Gubbins, S.; Paton, D.J.; Dekker, A.; Ludi, A.B.; Wilsden, G.; Browning, C.F.J.; Eschbaumer, M.; Barnabei, J.; Duque, H.; Pauszek, L.L.; King, D.P. Predicting cross-protection against foot-and-mouth disease virus strains by serology after vaccination. Front Vet. Sci. 2022, 9, 1027006. [Google Scholar] [CrossRef] [PubMed] [PubMed Central]
- Park, M.-Y.; Han, Y.J.; Choi, E.-J.; et al. “Post-vaccination Monitoring to Assess Foot-and-Mouth Disease Immunity at Population Level in Korea”. Front. Vet. Sci. 2021, vol.8, 673820. [Google Scholar]
- Choi, J.; Jo, H.J.; Jung, S.S.; Choi, J.; et al. “Evaluation of swine protection with foot-and-mouth disease O 1/Campos and O/Primorsky/2014 vaccines against the O Mya-98 lineage virus from East Asia”. Vaccine 2021, Vol. 39(12), 1701–1707. [Google Scholar] [CrossRef] [PubMed]
Figure 1.
Phylogenetic tree showing the genetic relationships of FMDV type O 2019–2024 isolates in Vietnam. Maximum Likelihood tree was constructed computing the evolutionary distances by Tamura 3-parameter model, based on the comparison of the complete region coding for VP1 protein, using the Mega program, version XII. Sequences obtained are indicated, together with their accession numbers (▲). Viruses used for comparisons were obtained from GenBank. Relevant lineages and topotypes are indicated with brackets. Scale bar refers to a phylogenetic distance of 0.1 nucleotide substitutions per site.
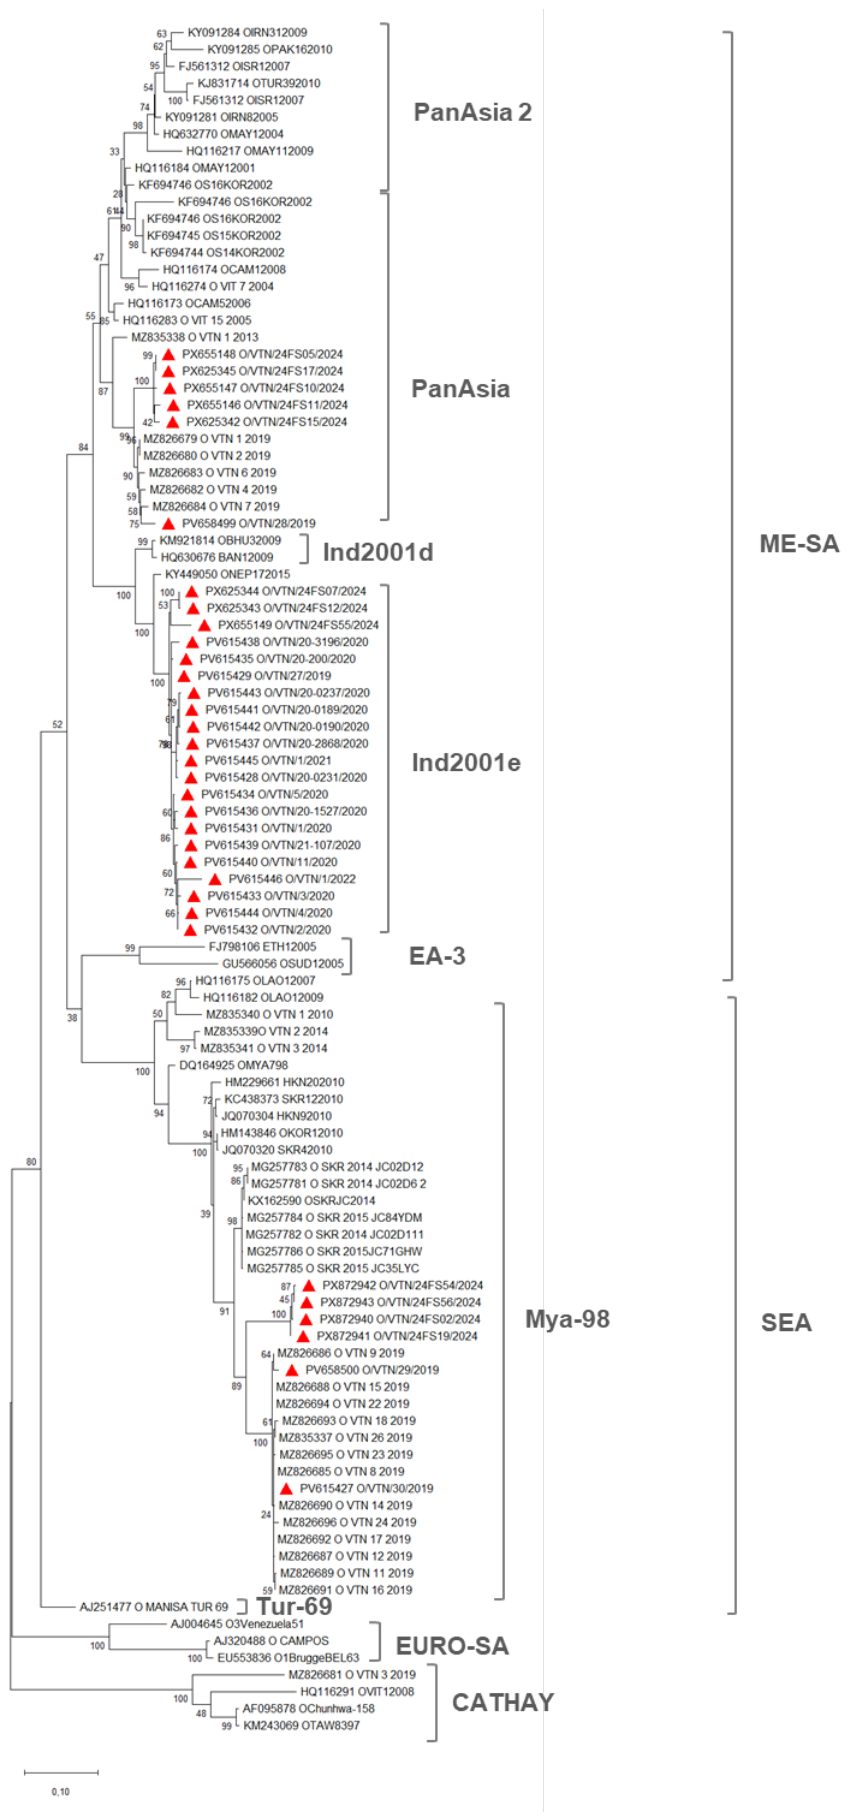
Figure 2.
Amino acid sequences of antigenic regions in VP1 of FMDVs. Amino acid alignment of VP1 sequences from Vietnamese FMDV serotype O isolates collected between 2019 and 2024, using the O1 Campos vaccine strain (AJ320488) as reference. Colored ▲ indicate the lineage assignment of each isolate: purple ▲ correspond to PanAsia isolates, light blue ▲ to Ind-2001 isolates, and green ▲ to Mya-98 isolates. Dots indicate amino acid residues identical to O1 Campos, whereas letters indicate amino acid substitutions. Highlighted boxes indicate antigenically relevant regions of VP1: the BC loop region (residues 40–60; orange), the GH loop region (residues 130–160; blue), the RGD motif involved in cell attachment (residues 145–147; red), and the C-terminal region (residues 200–211; green).
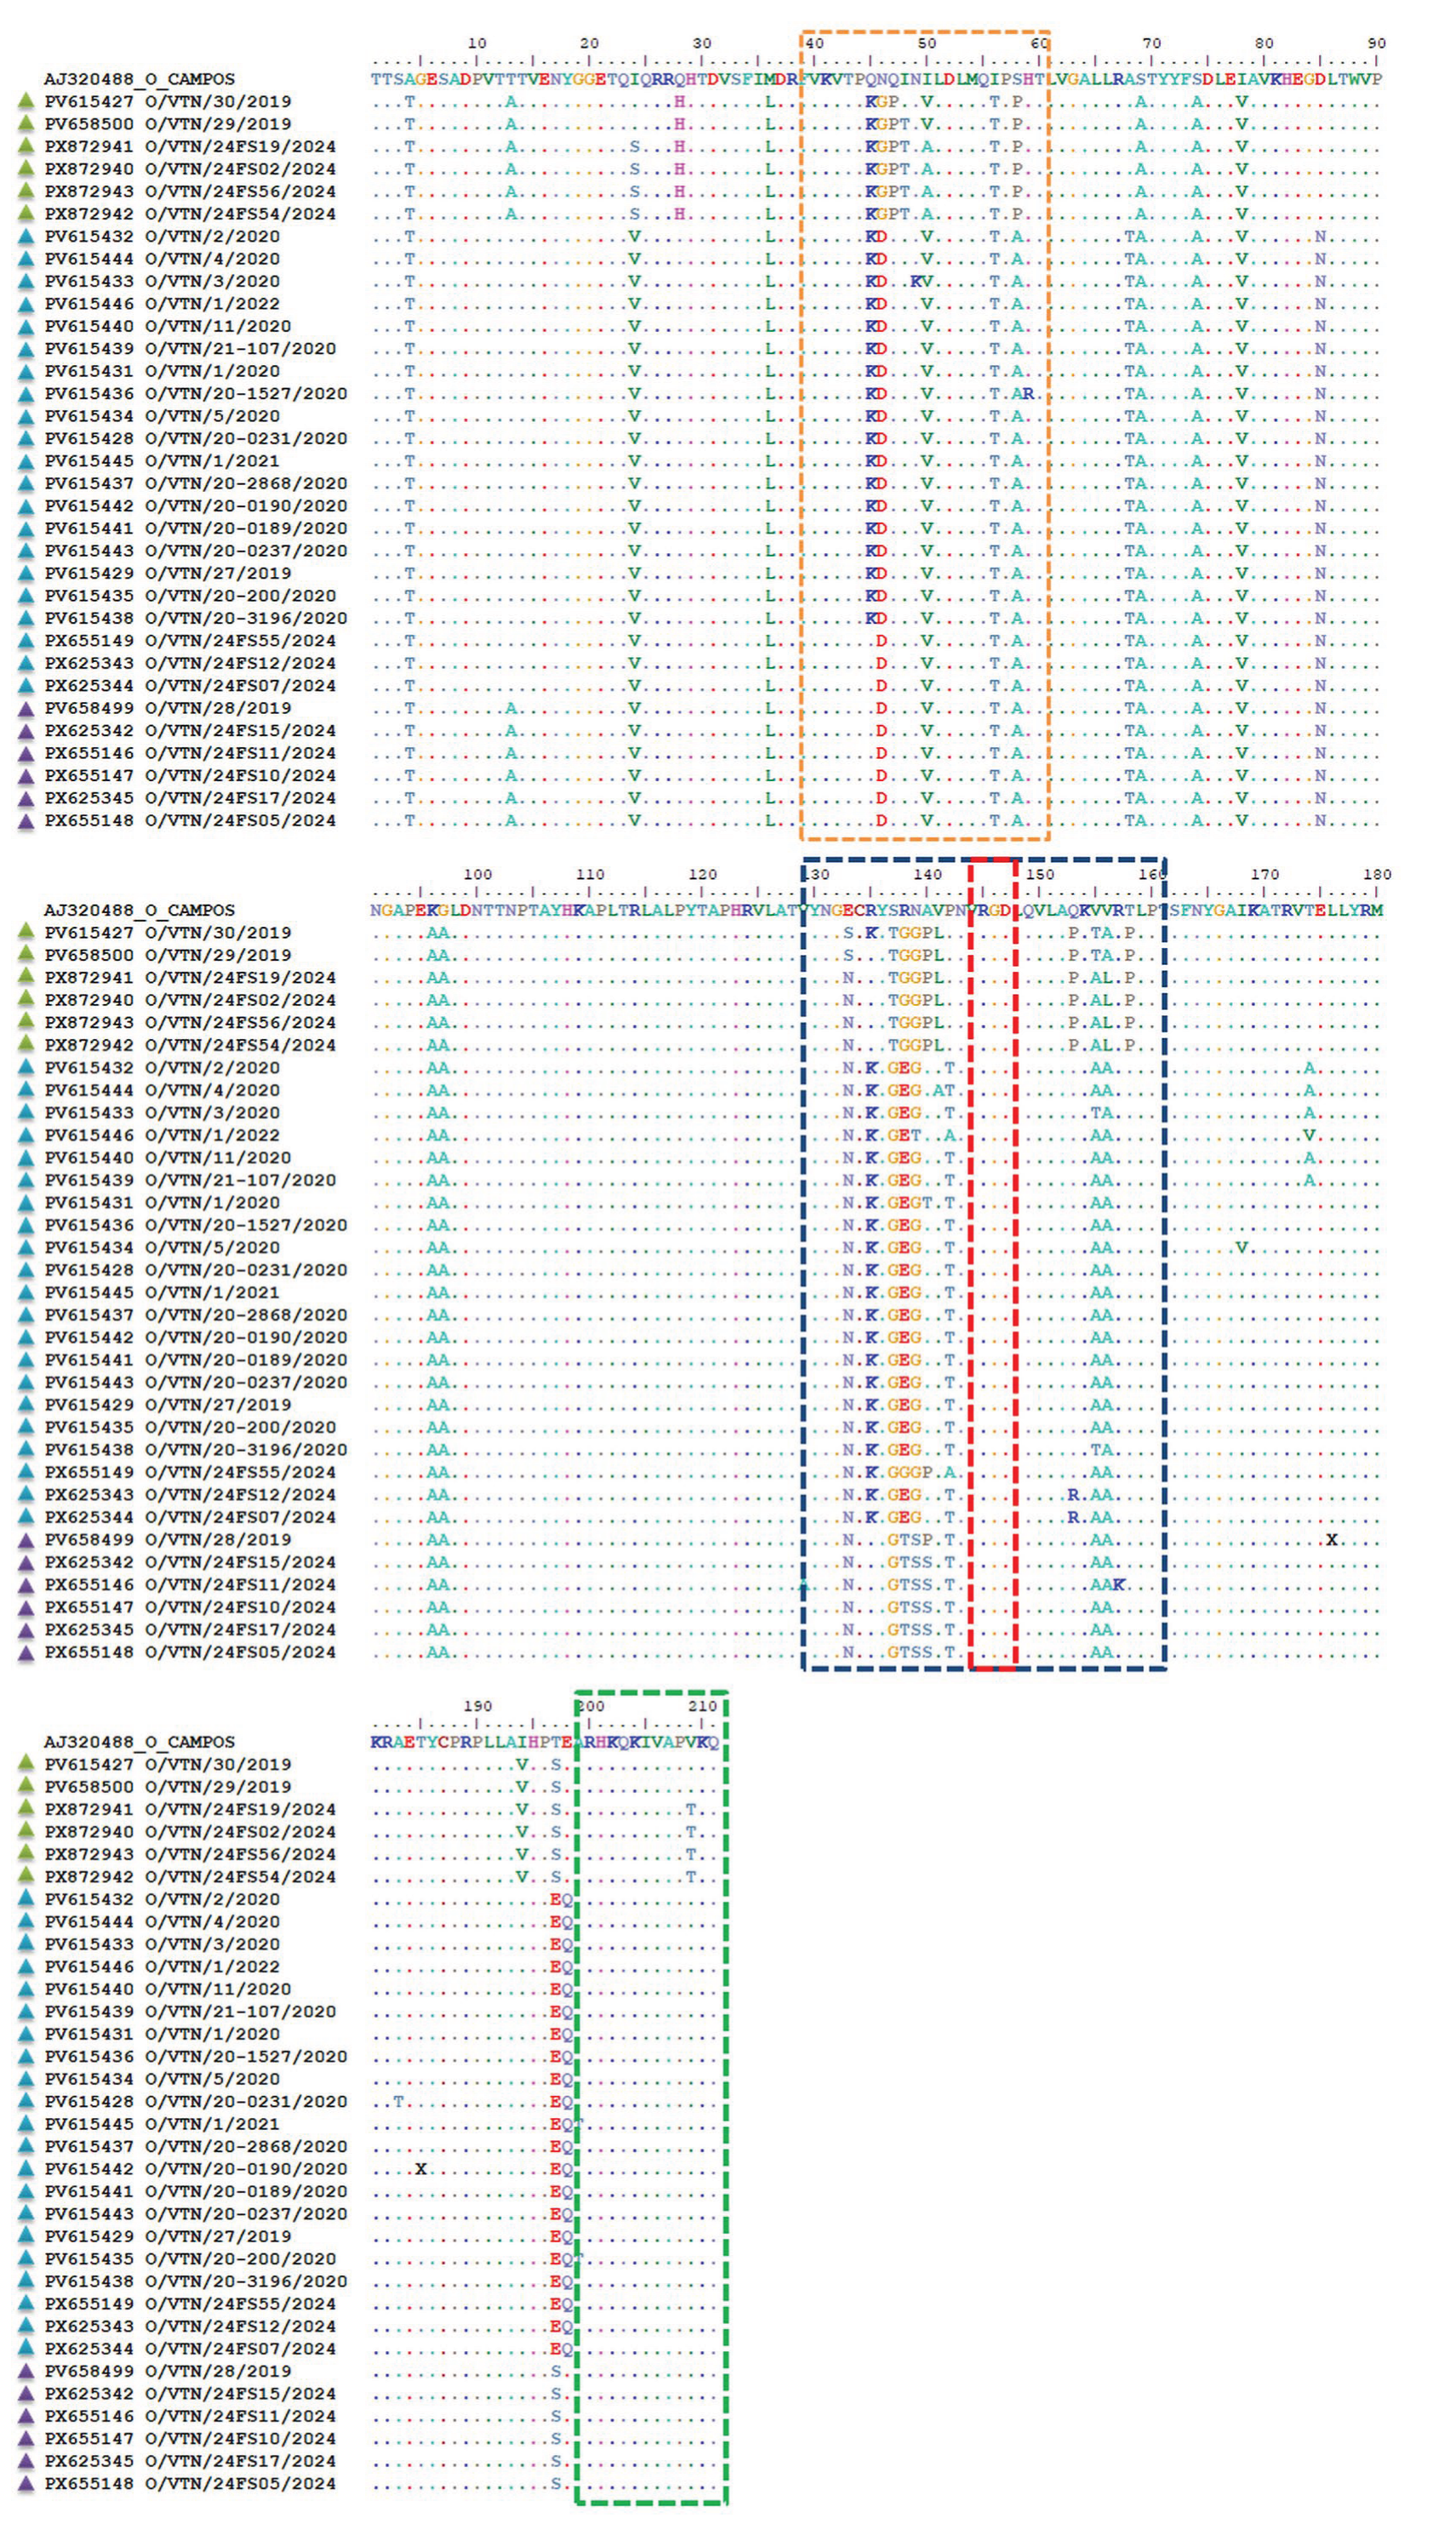

Table 1.
FMDV serotype O field isolates collected in Vietnam between 2019 and 2024, including accession number, province of origin, host species, and year of collection.
Table 1.
FMDV serotype O field isolates collected in Vietnam between 2019 and 2024, including accession number, province of origin, host species, and year of collection.
| Accession n. | Strain | Lineage | Topotype | Country | Year | Host |
|---|---|---|---|---|---|---|
| PV615446 | O/VTN/1/2022 | Ind2001e | ME-SA | Vietnam, Đồng Nai | 2022 | Cattle |
| PV615445 | O/VTN/1/2021 | Ind2001e | ME-SA | Vietnam, Trà Vinh | 2021 | Cattle |
| PV615444 | O/VTN/4/2020 | Ind2001e | ME-SA | Vietnam, Long An | 2020 | Cattle |
| PV615443 | O/VTN/20-0237/2020 | Ind2001e | ME-SA | Vietnam, Trà Vinh | 2020 | Cattle |
| PV615442 | O/VTN/20-0190/2020 | Ind2001e | ME-SA | Vietnam, Trà Vinh | 2020 | Cattle |
| PV615441 | O/VTN/20-0189/2020 | Ind2001e | ME-SA | Vietnam, Trà Vinh | 2020 | Cattle |
| PV615440 | O/VTN/11/2020 | Ind2001e | ME-SA | Vietnam, Nghệ An | 2020 | Cattle |
| PV615439 | O/VTN/21-107/2020 | Ind2001e | ME-SA | Vietnam, Quàng Ninh | 2020 | Cattle |
| PV615438 | O/VTN/20-3196/2020 | Ind2001e | ME-SA | Vietnam, Lạng Sơn | 2020 | Buffalo |
| PV615437 | O/VTN/20-2868/2020 | Ind2001e | ME-SA | Vietnam, Lạng Sơn | 2020 | Buffalo |
| PV615436 | O/VTN/20-1527/2020 | Ind2001e | ME-SA | Vietnam, Cao Bắng | 2020 | Buffalo |
| PV615435 | O/VTN/20-200/2020 | Ind2001e | ME-SA | Vietnam, Quàng Ninh | 2020 | Cattle |
| PV615434 | O/VTN/5/2020 | Ind2001e | ME-SA | Vietnam, Đồng Nai | 2020 | Cattle |
| PV615433 | O/VTN/3/2020 | Ind2001e | ME-SA | Vietnam, Vung Tàu | 2020 | Pig |
| PV615432 | O/VTN/2/2020 | Ind2001e | ME-SA | Vietnam, Tiên Giang | 2020 | Pig |
| PV615431 | O/VTN/1/2020 | Ind2001e | ME-SA | Vietnam, Bình Phuồc | 2020 | Cattle |
| PV615429 | O/VTN/27/2019 | Ind2001e | ME-SA | Vietnam, Bình Phuồc | 2019 | Cattle |
| PV615428 | O/VTN/20-0231/2020 | Ind2001e | ME-SA | Vietnam, Trà Vinh | 2020 | Cattle |
| PX625344 | O/VTN/24FS07/2024 | Ind2001e | ME-SA | Vietnam, Điện Biên | 2024 | Buffalo |
| PX625343 | O/VTN/24FS12/2024 | Ind2001e | ME-SA | Vietnam, Sơn La | 2024 | Cattle |
| PX655149 | O/VTN/24FS55/2024 | Ind2001e | ME-SA | Vietnam, Bắc Kạn | 2024 | Buffalo |
| PV658499 | O/VTN/28/2019 | PanAsia | ME-SA | Vietnam, Quàng Ninh | 2019 | Buffalo |
| PX655148 | O/VTN/24FS05/2024 | PanAsia | ME-SA | Vietnam, Điện Biên | 2024 | Buffalo |
| PX655147 | O/VTN/24FS10/2024 | PanAsia | ME-SA | Vietnam, Sơn La | 2024 | Cattle |
| PX655146 | O/VTN/24FS11/2024 | PanAsia | ME-SA | Vietnam, Sơn La | 2024 | Cattle |
| PX625342 | O/VTN/24FS15/2024 | PanAsia | ME-SA | Vietnam, Sơn La | 2024 | Cattle |
| PX625345 | O/VTN/24FS17/2024 | PanAsia | ME-SA | Vietnam, Lào Cai | 2024 | Cattle |
| PV615427 | O/VTN/30/2019 | Mya-98 | SEA | Vietnam, Cà Mau | 2019 | Pig |
| PV658500 | O/VTN/29/2019 | Mya-98 | SEA | Vietnam, Kon Tum | 2019 | Cattle |
| PX872940 | O/VTN/24FS02/2024 | Mya-98 | SEA | Vietnam, Hòa Bình | 2024 | Pig |
| PX872941 | O/VTN/24FS19/2024 | Mya-98 | SEA | Vietnam, Yên Bái | 2024 | Pig |
| PX872942 | O/VTN/24FS54/2024 | Mya-98 | SEA | Vietnam, Lào Cai | 2024 | Cattle |
| PX872943 | O/VTN/24FS56/2024 | Mya-98 | SEA | Vietnam, Vĩnh Phúc | 2024 | Pig |
Table 2.
VNT titer (Log10) and r1 value of O1 Campos calculated for each field strain. The media of three repetitions and their standard deviation is presented.
Table 2.
VNT titer (Log10) and r1 value of O1 Campos calculated for each field strain. The media of three repetitions and their standard deviation is presented.
| Accession n. | Sample | Titer | r1 value | SD |
|---|---|---|---|---|
| PV615446 | O/VTN/1/2022 | 2,51 | 0,79 | 0,12 |
| PV615445 | O/VTN/1/2021 | 2,34 | 0,75 | 0,21 |
| PV615444 | O/VTN/4/2020 | 2,67 | 1,00 | 0 |
| PV615443 | O/VTN/20-0237/2020 | 2,08 | 0,97 | 0,05 |
| PV615442 | O/VTN/20-0190/2020 | 2,16 | 1,00 | 0 |
| PV615441 | O/VTN/20-0189/2020 | 1,92 | 0,56 | 0,16 |
| PV615440 | O/VTN/11/2020 | 2,26 | 0,98 | 0,03 |
| PV615439 | O/VTN/21-107/2020 | 2,18 | 1,00 | 0 |
| PV615438 | O/VTN/20-3196/2020 | 2,09 | 1,00 | 0 |
| PV615437 | O/VTN/20-2868/2020 | 2,13 | 0,88 | 0,13 |
| PV615436 | O/VTN/20-1527/2020 | 1,91 | 0,44 | 0,06 |
| PV615435 | O/VTN/20-200/2020 | 1,63 | 0,29 | 0,11 |
| PV615434 | O/VTN/5/2020 | 1,65 | 0,30 | 0,1 |
| PV615433 | O/VTN/3/2020 | 1,81 | 0,49 | 0,18 |
| PV615432 | O/VTN/2/2020 | 2,62 | 1,00 | 0 |
| PV615431 | O/VTN/1/2020 | 2,52 | 1,00 | 0 |
| PV615429 | O/VTN/27/2019 | 2,24 | 0,88 | 0,17 |
| PV615428 | O/VTN/20-0231/2020 | 2,15 | 0,90 | 0,1 |
| PX625344 | O/VTN/24FS07/2024 | 1,51 | 0,37 | 0,04 |
| PX625343 | O/VTN/24FS12/2024 | 1,50 | 0,36 | 0,09 |
| PX655149 | O/VTN/24FS55/2024 | 1,53 | 0,39 | 0,07 |
| PV658499 | O/VTN/28/2019 | 2,28 | 1,00 | 0 |
| PX655148 | O/VTN/24FS05/2024 | 1,74 | 0,40 | 0,14 |
| PX655147 | O/VTN/24FS10/2024 | 1,75 | 0,64 | 0,14 |
| PX655146 | O/VTN/24FS11/2024 | 1,62 | 0,49 | 0,16 |
| PX625342 | O/VTN/24FS15/2024 | 1,50 | 0,36 | 0,06 |
| PX625345 | O/VTN/24FS17/2024 | 1,7 | 0,57 | 0,09 |
| PV615427 | O/VTN/30/2019 | 1,97 | 0,76 | 0,12 |
| PV658500 | O/VTN/29/2019 | 2,21 | 0,95 | 0,08 |
| PX872940 | O/VTN/24FS02/2024 | 1,50 | 0,36 | 0,11 |
| PX872941 | O/VTN/24FS19/2024 | 1,50 | 0,36 | 0,06 |
| PX872942 | O/VTN/24FS54/2024 | 1,74 | 0,39 | 0,07 |
| PX872943 | O/VTN/24FS56/2024 | 1,50 | 0,24 | 0,05 |
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (http://creativecommons.org/licenses/by/4.0/).
Copyright: This open access article is published under a Creative Commons CC BY 4.0 license, which permit the free download, distribution, and reuse, provided that the author and preprint are cited in any reuse.