

Submitted:
10 September 2026
Posted:
11 September 2026
You are already at the latest version
Abstract
Phragmites australis (common reed) is a resilient wetland species providing key ecosystem services, including carbon sequestration. However, its carbon storage potential in hyper-arid environments remains insufficiently quantified. This study develops an integrated framework combining destructive sampling and remote sensing to assess biomass distribution and carbon stocks in Oman. Results show that destructively measured AGB correlates only weakly with reed height (R² = 0.15), indicating that height alone is not a reliable standalone predictor of biomass in this system; an initially high fit (R² ≈ 0.99) reflected the mathematical dependence of the height-based allometric equations on their own input variable rather than genuine predictive validity. While predictive models based on dry biomass and TOC showed moderate to low performance (R² < 0.16), vegetation indices derived from remote sensing demonstrated high accuracy in estimating spatial biomass variability. Carbon stock estimates ranged between ~0.36 and 1.95 kg/m² depending on the method used. While localized allometric models showed limited predictive power due to high variability in tiller density, vegetation spectral indices demonstrated high accuracy (R² = 0.78), highlighting remote sensing as a viable tool for spatial carbon assessment in arid wetland ecosystems. These findings highlight the potential of integrating field-based and remote sensing approaches to improve carbon accounting in arid wetlands. The study provides a scalable framework for ecosystem-based carbon assessment and supports the role of P. australis as a nature-based solution for climate mitigation in water-stressed regions.
Keywords:
Phragmites australis
; above ground biomass
; carbon sequestration
; destructive method
; GIS
; remote sensing
1. Introduction
Phragmites australis, commonly known as common reed grass, is a typical wetland vegetation known for its aggressive invasiveness in regional ecosystems. This robust, herbaceous, perennial wetland plant plays a crucial role in wet- land ecosystem services, such as carbon storage, nutrient cycling, and heavy metal absorption [1]. This plant exhibits rapid growth potential, capable of reaching heights of up to 5 meters [1]. Once established, it rapidly forms dense mono- typic stands through aerial seed dispersal and extensive rhizome networks [2]. Phragmites australis can quickly dominate invaded areas due to its fast growth rates [2], tolerance to salinity [3], and exploitation of anthropogenic impacts on wetlands [4]. In North America, Phragmites is particularly recognized as an aggressive invader in regional ecosystems [5]. Hence, to uphold the diversity and resilience of wetland ecosystems, it is crucial to regulate and manage the aboveground biomass (AGB) of common reed. An essential aspect of this management involves effectively estimating the AGB of common reed. Despite extensive global research on wetland carbon dynamics, limited studies have quantified biomass and carbon sequestration of Phragmites australis under hyper-arid conditions such as those in Oman. Furthermore, integration of destructive sampling with remote sensing for scalable carbon estimation remains underdeveloped in such environments.
On other hand, Phragmites australis presents significant long-term carbon (C) reservoirs that accumulate atmospheric carbon at annual rates comparable to terrestrial forest types despite their limited global coverage [6,7]. These carbon stocks and exchanges in intertidal areas are collectively termed “coastal wetland blue carbon” [8]. Specifically, tidal marsh carbon stocks sequester carbon at average rates of 1–2 Mg C per hectare per year (IPCC, 2014), although they are undergoing con- version to open water or other land cover types at global rates of 1–2% [9,10].
Phragmites australis plays a vital role in up- holding the ecological balance of wetlands and offering various ecosystem services, including water purification, habitat provision, biodiversity conservation, and carbon sequestration [11,12]. Through photosynthesis, during its growth phase, Phragmites australis can assimilate significant amounts of carbon, thereby aiding in mitigating carbon emissions and promoting carbon neutrality [13]. Biomass, which refers to the dry weight of the living organic part of Phragmites australis serves as a crucial indicator of its capacity for carbon sequestration [14]. With growing concerns about climate change due to excessive car- bon emissions, there is a rising interest in estimating the biomass and carbon sequestration potential of wetland plants like Phragmites australis. This attention aims to support carbon management efforts and work towards achieving carbon neutrality [15,16,17].
The conventional method of measuring plant biomass involves on-site sampling at the plot level, a process that is known to be time- consuming, labor-intensive, and sometimes im- practical due to challenges related to site accessibility [18]. Besides field sampling, a growth dynamics model for vegetation has been devised to estimate biomass. These models are grounded in the eco-physiological processes of the plants they model, such as photosynthesis, respiration, and mortality. This approach enables a more frequent measurement of plant biomass, like on a daily basis, providing a more detailed understanding of biomass variation and carbon sequestration capacity [19,20,21]. Asaeda and Karunaratne [20] were pioneers in establishing a growth dynamics model for Phragmites australis, focusing on key variables like shoot biomass, inflorescence, roots, old rhizomes, and new rhizomes. They used mathematical relationships to quantify plant growth by considering photosynthesis, respiration, mortality, and material translocation between organs, effectively reflecting the growth dynamics of Phragmites australis [13,20]. Through specific calibration and validation, this model has been employed in various case studies to explore Phragmites australis growth dynamics [13,22]. For example, [13] studied the meteorological effects on Phragmites australis growth in the Scheldt estuary, while [22] simulated biomass and carbon sequestration in a Mediterranean eutrophic lake. Environmental factors like latitude and nutrient availability have been parameterized in these models to simulate plant growth traits and their response to environmental changes, aiding in carbon management [19,23,24]. However, the development and application of these growth models depend on field biomass data for necessary calibration and validation [25].
Plants absorb and distribute both macro- and micro-nutrients within their tissues, facilitating the transfer of these nutrients among various plant organs. This internal cycling of nutrients is significant in wetland ecosystems. Notably, high- yield plants such as Phragmites australis can extract substantial quantities of nutrients from their surroundings on an annual basis. As a result, wetland plants are employed to mitigate nutrient levels in domestic, industrial, and agricultural wastewater streams [26,27].
Remote sensing is an advantageous method for monitoring vegetation. Various types of remote sensing data, such as optical images, light detection and ranging (LiDAR) point cloud data, and synthetic aperture radar (SAR) data, have been extensively utilized to quantify above- ground biomass (AGB) of different plants [28]. Through establishing relationships between re- mote sensing data, like reflectance and vegetation indices, and actual biomass collected in the field, remote sensing technology enables rapid and accurate estimation of AGB [29,30]. This technology proves particularly beneficial in wetland environments due to their remote and hard-to- access nature, covering vast areas [31]. For in- stance, [32] demonstrated the capability of hyper- spectral compact airborne spectrographic imager data to retrieve the AGB of Phragmites australis in the Zhangye National Wetland Park, China, while [5] developed an empirical model for AGB retrieval of these vegetations in Dafeng, China. Therefore, biomass data acquired through remote sensing serves as a valuable resource for calibrating and validating plant growth dynamics models. In our investigation, we found that there is a lack in establishing a framework to assess the significance of Phragmites australis (Reed Grass) in carbon sequestration and phytoremediation within the hyper arid region including Oman. Hence, the main objective of this study was to evaluate biomass and carbon dynamics of Phragmites australis in arid environments by addressing four key aspects: (i) quantifying the distribution of biomass and carbon among different plant organs, (ii) comparing aboveground biomass (AGB) estimates derived from dry biomass and Total Organic Carbon (TOC) approaches, (iii) developing a localized allometric model for reliable carbon estimation under arid conditions such as Oman, and (iv) assessing the potential of remote sensing techniques for scalable estimation of biomass and carbon sequestration.
2. Results
Phragmites australis, commonly known as common reed, is a perennial grass species widely distributed in wetland ecosystems worldwide. It exhibits remarkable adaptability to various environmental conditions, including freshwater and brackish marshes, riverbanks, and disturbed habitats. Phragmites australis plays a significant ecological role in wetlands and offers various ecosystem services, including carbon sequestration and aboveground biomass production.
The study involved a meticulous process of collecting data on reed biomass using destructive sampling methods (Figure 1). The aboveground shoots of reedgrass were systematically collected from approximately 12 selected locations within the designated plant area to facilitate an in-depth analysis of carbon stock. The collection area for each sample encompassed a 1 1 square meter plot. To ensure accurate measurement, proper care was taken to obtain representative samples from various parts of the reedgrass population.
2.1. Carbon Stock Comparison
Upon collection, the reedgrass samples under- went a meticulous process for carbon stock analysis. The first step involved subjecting the samples to oven drying at a controlled temperature of 105 C duration of 48 hours. This process facilitated the removal of moisture and ensured the determination of the dry-weight biomass of the reedgrass shoots. To prepare the samples for subsequent analysis, the dried reedgrass shoots were carefully cut and finely ground until they could pass through a 60-mesh stainless steel sieve. This sieving process helped to achieve a consistent particle size for the samples, which is crucial for reliable and accurate carbon analysis. The processed reedgrass samples were then stored in specialized glass vials, which were placed in a desiccator to maintain a controlled and moisture-free environment. This storage condition was essential to preserve the integrity and stability of the samples before carbon analysis.
The concentrations of Total Organic Carbon (TOC) in the reedgrass samples were quantified using a TOC analyzer, a widely recognized and reliable instrument for determining carbon content. This analysis allowed for precise measurement of the TOC levels, an important parameter for assessing the carbon stock.
The carbon stock in the reedgrass samples was subsequently calculated based on the TOC con- centration, expressed as a percentage, multiplied by the corresponding dry weight of the sample. The resulting carbon stock values were then ex- pressed in grams per square meter (g m 2), providing a quantitative measure of the carbon content within the reedgrass ecosystem. By employing this rigorous methodology, encompassing sample collection, preparation, analysis, and calculation, a comprehensive evaluation of the carbon stock in the reedgrass samples was accomplished, allowing for a more profound understanding of the carbon dynamics within the studied ecosystem.
The results are presented in a structured manner to highlight biomass distribution, carbon stock estimation approaches, model performance, and the integration of remote sensing techniques for biomass assessment. As shown in Figure 2, a visual representation of the complete destructive site process employed in this study. The process encompasses several crucial steps, including pre-cutting measurements, comprehensive weight determination of all reed grass plot components, systematic sample collection, precise acquisition of the fresh weight of the samples, and subsequent controlled drying of the samples within the controlled environment of the university drying laboratory. This visual depiction serves as a valuable guide, providing a comprehensive overview of the step-by-step procedures involved in the site process leading up to the drying phase. By incorporating this visual representation in our academic paper, readers can easily grasp the procedural flow and understand the meticulous approach taken to ensure accurate measurements and consistent drying process.
Illustrates data pertaining to various plot numbers within the designated site, detailing their dimensions, reed heights, reed count per plot, reed plot weight, as well as the fresh and dry weights of samples gathered from each plot. The plots are sequentially numbered from 1 to 12, each measuring 1 meter by 1 meter, and are systematically sampled surrounding the reed oasis area.
For clarity, four related but distinct variables are used throughout this section and are defined here: (1) fresh weight (kg/plot), the raw weight of harvested reed material recorded in the field before drying (Table 1); (2) dry weight (g), the weight of the oven-dried subsample used to derive the wet-dry ratio (Table 1); (3) aboveground biomass, AGB (kg/m²), the dry-mass-equivalent biomass per unit area, obtained either from the dry-weight ratio approach or converted from the TOC approach (Table 2); and (4) carbon stock (kg/m²), the carbon content per unit area, derived by applying the carbon conversion factor to AGB (dry-ratio approach) or measured directly via TOC analysis. Values quoted below are labelled explicitly with the corresponding variable and unit to avoid the ambiguity between these related quantities.
Aboveground biomass varied significantly across the 12 plots (Table 1), with reed height ranging from 2.2 to 4.3 m. Notably, tiller density did not correlate linearly with aboveground biomass (AGB), as Plot 1 exhibited the highest tiller density (214 tillers) but only a moderate raw fresh weight (3.7 kg/plot, equivalent to 1.81 kg/m² AGB from the dry-ratio approach) compared to Plot 9 (73 tillers, 7.5 kg/plot fresh weight, equivalent to 3.91 kg/m² AGB).
Furthermore, Table 1 provided presents data related to two different approaches for estimating carbon stocks in reed plots. The first approach is the Dry Weight Ratio Approach, which includes the reed wet-dry ratio, reed aboveground biomass (AGB) in kilograms per square meter (kg/m2) from the dry weight ratio where the reed carbon stock in kg/m2 is also calculated. The second approach is the TOC (Total Organic Carbon) Approach, which includes the TOC percentage in the collected sample plots.
For each plot, the values for the different parameters in both approaches were calculated. The reed wet-dry ratio ranges from 0.306 to 0.744, indicating the moisture content of the reed samples. The reed AGB from the dry weight ratio varies between 1.51 kg/m2 and 3.91 kg/m2, while the reed carbon stock from the dry weight ratio ranges from 0.75 kg/m2 to 1.95 kg/m2. In the TOC Approach, the TOC percentage ranges from 10.8% to 25.2%, representing the proportion of carbon content in the reed samples. The carbon stock from the TOC Analyzer varies between 0.3584 kg/m2 and 1.3125 kg/m2.
This data allows for comparisons between the two approaches and the assessment of carbon stocks in the reed plots using different estimation methods. Further analysis could involve evaluating the consistency or discrepancies between the results obtained from the Dry Weight Ratio Approach and the TOC Approach and discussing the implications for carbon stock assessments in reed ecosystems (Table 2).
Total Organic Carbon (TOC) method: The TOC method estimates biomass by determining the amount of organic carbon present in the plant material. This method involves collecting plant samples, drying them to remove moisture, and then analyzing the carbon content using laboratory techniques such as elemental analysis or combustion.
The TOC method provides an indirect estimation of biomass based on the assumption that a certain proportion of the plant’s organic carbon is derived from biomass. The actual proportion can vary depending on the plant species and environ- mental factors, so it is essential to calibrate the method for specific ecosystems.
Dry-to-wet ratio method: The dry-to-wet ratio method estimates biomass by determining the ratio of dry weight to wet weight of the plant material. It involves collecting fresh plant samples, weighing them immediately (wet weight), and then drying them in an oven until a constant weight is achieved (dry weight). The biomass is calculated by multiplying the wet weight by the dry-to-wet ratio.
The dry-to-wet ratio method assumes that the water content of the plant material is relatively constant, and the difference between wet weight and dry weight is mainly due to water loss during drying. This method can provide a quick estimation of biomass in the field, but it may introduce some errors if there are significant variations in water content among samples or if the water content changes during the drying process.
Both methods have their advantages and limitations, and the choice of method depends on the specific research objectives, available resources, and environmental conditions. It is always important to consider the specific characteristics of the plant species and ecosystem being studied and to validate the chosen method against ground truth measurements whenever possible.
Figure 3 presents a visual snapshot of the destructive sampling process conducted within the reed grass oasis, showcasing the 12 plots that were analyzed. The figure provides a visual representation of the in-situ measurements taken at each plot, including the number of reeds present, the weight of the reed plot, and the height of the reeds. This visualization offers a concise overview of the collected data, enabling a comprehensive understanding of the distribution and characteristics of the reed grass within the studied area. Figure 3 shows the spatial arrangement and quantitative measurements associated with the reed grass plots, enhancing the clarity and comprehensiveness of our research findings.
Figure 4 and Figure 5 provide a comparative analysis of the aboveground biomass (AGB) of Phragmites australis across 12 plots within the oasis. These figures showcase the comparison between two distinct approaches used for calculating AGB, despite their differences in methodology. Interestingly, the results obtained from both approaches demonstrate a remarkable degree of similarity, indicating a high level of agreement. Furthermore, these findings align closely with previous studies conducted on Phragmites australis, as demonstrated in Table 3. The inclusion of Figure 4 and Figure 5 enables a visual representation of the AGB comparisons, reaffirming the consistency and reliability of our findings, while also highlighting the broader consistency with prior research on Phragmites australis.
Figure 6 illustrates the relationship between the lab-calculated dry weight of the reed grass samples and the corresponding fresh-dry weight (moisture loss) over a specific timeframe, measured in grams. The findings indicate a noticeable reduction in moisture content occurring over an approximate duration of 8 days. These results highlight the rapid loss of moisture from the reed grass samples, indicating lower carbon sequestration capacity in non-woody plant species. This observation suggests that the relatively faster drying process in non-woody plants leads to reduced moisture content and potentially lower carbon storage compared to woody plants.
Figure 7 presents the values of three sample batches comprising 12 plots each, in relation to the output of total organic carbon expressed as a percentage (%). The figure provides an overview of the correlation between the sample batches and their corresponding plots. Notably, the results reveal a consistent correlation value across all batches and similar plots.
Figure 8 illustrates the carbon stock estimates across the 12 plots using two different approaches: the dry/fresh ratio method and the total organic carbon (TOC) approach. Although the values obtained from these approaches differ slightly, the discrepancies are minimal. Moreover, it is important to note that the TOC approach specifically calculates the content of organic carbon, providing a focused estimate in comparison to the broader carbon stock estimation using the dry/fresh ratio method. This supports the reliability and robustness of our findings, highlighting the relatively small variations and the specific focus on organic carbon content offered by the TOC approach.
2.2. Model Performance
The central aim of the reeds model’s evaluation fitting was to thoroughly assess the predictive precision of the ultimate selected models when estimating individual aboveground biomass (AGB) for reeds. To achieve this objective, the fitting dataset was employed, which contains relevant measurements and data pertaining to the target reed population. The use of this dataset allowed for a meticulous evaluation of the models’ performance and their capacity to accurately estimate the AGB of reeds oasis.
The first approach involved utilizing the dry- to-fresh ratio method, which entails quantifying biomass based on the weight ratio of dried reed samples to their corresponding fresh weight. The second approach was the Total Organic Carbon (TOC) method, which involves estimating AGB by measuring the total organic carbon content of reed samples (Figure 9 and Figure 10 and Figure 11). In addition to these two approaches, the study also incorporated the findings from Conti et al.’s (2019) research on plants like reeds. Conti et al.’s study, which explored biomass estimation in analogous plant species, served as a valuable reference point and benchmark for comparing the performance of the dry-to-fresh ratio and TOC methods when ap- plied to reeds.
Through a meticulous examination of both the dry-to-fresh ratio and TOC methods, along with insights gleaned from Conti study, the researchers sought to gain a comprehensive understanding of the most effective and accurate approach for estimating the aboveground biomass of reeds. By comparing these methodologies, this study aimed to contribute valuable insights to the field of wetland vegetation biomass estimation and advance knowledge in ecological modelling.
The subsequent matrix presents a comprehensive analysis of the correlation between the responses, focusing on aboveground biomass (AGB) or its natural logarithm (LN(AGB)), and the calculated predictors for reeds. The predictors examined include reed height (measured in meters), fresh weight (measured in kilograms per square meter), and the number of reeds stands per unit area of one square meter (Figure 12, Figure 13 and Figure 14). The matrix results unveil a significant correlation between the [38] study and the correlated regression equation, particularly concerning the reed height predictor. This finding indicates a strong alignment between the outcomes of the [38] study and the regression equation, specifically when estimating reed height.
However, the calculated aboveground biomass (AGB) obtained from both approaches showed notably weak correlations with the predictors of reed parameters (height, weight, and reed number). The exceptions to this were the calculated dry AGB, which demonstrated a commendable correlation with the reed weight predictor only. These correlation findings provide valuable insights into the efficacy of the applied methodologies for estimating aboveground biomass in reeds. The notable correlation with reed weight in the context of calculating dry AGB suggests a potential avenue for enhancing biomass estimation accuracy. Nonetheless, the observed weak correlations between the predictors and the calculated AGB highlight the complexity of the biomass estimation process for reeds. This detailed analysis aims to contribute significant knowledge to the field of vegetation biomass estimation and improve ecological modelling practices.
In the pursuit of novel models for estimating aboveground biomass (AGB) of Phragmites australis (Reed grass), we integrated equations from a prior study conducted by [38] with regression model equations focused on destructive correlation of Phragmites australis (Reed grass) data, as documented in Table 4. Subsequently, stepwise regression was applied to a dataset encompassing measurements obtained from 12 distinct plots of Phragmites australis (Reed grass). A comprehensive evaluation of the newly devised models was undertaken, utilizing prominent indicators such as R2 and P-Value to assess their efficacy.
Integral to the model construction, we included essential reed variables, namely height, weight of fresh reeds, and the number of reeds per plot. This strategic incorporation of these variables served to enrich the analytical framework and enhance the model’s predictive capacity. Among the various models explored for AGB estimation in Phragmites australis (Reed grass), two height-based logarithmic models stood out as candidates for further evaluation: Model#1, applied directly from the published allometric equation of Conti et al. (2019) for reed-like species, and Model#2, a recalibration of that equation’s intercept to align with this study’s TOC-based carbon estimates, while retaining the same height-scaling slope. Because both equations compute AGB as a direct mathematical function of height, each shows a strong internal correlation with reed height by construction; this reflects consistency with their own input variable rather than independent validation against the destructively measured AGB values collected in this study (see Section 2.2 and Discussion).
It is worth noting that the AGB values yielded of model#1 were in closer agreement with the calculated values from the harvested samples of the fresh-to-dry approach, as depicted in Figure 15. On the other hand, the new novel modified models (Model#2) derived from Model#1 demonstrated favorable fit values for crucial indicators such as R2 and P-Value, as evident in Table 4, Figure 15 and Figure 16.
By encompassing characteristics of both the fresh-to-dry and Total Organic Carbon (TOC) calculation approaches, Model#1 and Model#2 occupied an intermediate position, ensuring that the results for all plots were suitably positioned between these two studies calculated approaches. This unique feature of the models contributed to their suitability and versatility in accommodating varying conditions and improved the overall accuracy of AGB estimation for Phragmites australis (Reed grass) vegetation as shown in Figure 15. However, with evaluation of two models, model two does not show a good value for MAE, MAPE, RE and RMSE compared to model one.
The final regression equations presented provide useful methods for estimating aboveground biomass (AGB) in Phragmites australis oasis environments, as detailed in Table 5. By evaluating correlation indicators such as MAE, MAPE, R2 and RMSE, the Model#1 regression equations are identified as the optimal choice due to their high R2 and low errors in MAE, MAPE, RE and RMSE, making it the best fit for estimating the AGB of Phragmites australis (Reed grass). These results span various ecological contexts, enhancing the understanding of wet- land vegetation biomass and advancing ecological modeling practices.
Table 5 displays a comprehensive overview of our novel regression model devised for the estimation of aboveground biomass (AGB) within Phragmites australis (commonly known as Reed grass) populations. This model is the result of a meticulous statistical correlation regression analysis conducted across specific targeted locations. Drawing insights from prior research endeavors and on-the- ground measurements, these models incorporate a spectrum of variables and anticipated outcomes. They thus serve as invaluable tools for both practitioners and researchers seeking precise quantification of aboveground biomass within these plant communities. Furthermore, these models adopt a holistic approach by encompassing both total organic carbon and dry biomass methodologies.
Through this study, we contribute to the evolving comprehension of carbon sequestration dynamics and biomass assessment methodologies across di- verse ecological contexts. Such insights are pivotal for advancing ongoing initiatives in climate change research and ecological modeling endeavors.
The performance evaluation of two models for estimating dry biomass and Total Organic Carbon (TOC) is shown in Table 6. For dry biomass, both models exhibit low R2 values (Model-1: 0.156, Model-2: 0.152), indicating weak predictive power. However, Model-1 demonstrates lower errors (MAE = 0.193, RMSE = 0.248) and better relative errors (-3.8%) compared to Model-2 (MAE = 0.461, RMSE = 0.522, RE = -46.1%), Model-1 demonstrates slightly higher reliability, supported by the closer agreement of AGB values shown in Figure 15.
In TOC estimation, both models also show low R2 values (Model-1: 0.024, Model-2: 0.026), indicating poor model fit. Model-2 performs better with lower MAE (0.217) and RMSE (0.313), along with a lower MAPE (124.7%), compared to Model-1 (MAE = 0.478, RMSE = 0.508, MAPE = 463.4%). Overall, both models struggle with accurate predictions, but Model-1 performs relatively better for dry biomass, while Model-2 is more reliable for TOC estimation.
The very poor fit of the TOC-based models (R² = 0.024–0.026, MAPE up to 463%) warrants explanation rather than being reported as a standalone predictive result. TOC% is a compositional laboratory measurement of organic carbon content and is not mechanistically linked to the morphological predictors (height, tiller density, fresh weight) used in these regressions; with only 12 plots and no expected causal relationship between TOC% and plant size, a near-zero R² is the expected outcome rather than an anomaly. We therefore do not recommend the TOC-based allometric models as predictive tools for this dataset. Their value lies instead in independently verifying the carbon-fraction estimate (Table 2) and in flagging cases where the dry-weight-ratio approach may be biased by inorganic carbonate content in these alkaline soils; we have revised the framing throughout the manuscript accordingly.
2.3. Remote Sensing Validation
Remote sensing-derived vegetation indices demonstrated strong potential for estimating biomass at larger spatial scales. Significant correlations were observed between selected vegetation indices and field-measured biomass, confirming the feasibility of integrating remote sensing with field data. This approach supports scalable carbon assessment and enhances monitoring capabilities in arid wetland ecosystems. This investigation involved a comprehensive evaluation of spectral reflectance and vegetation indices (VIs) for reed plants across multiple model combinations. The integration of multi-band reflectance data with selected VIs resulted in a high level of precision in estimating Above-Ground Biomass (AGB). As summarized in Table 7 and visually validated in Figure 17, both Model 1 and Model 2, which incorporate satellite imagery, achieved the highest estimation accuracy for reed grass. Specifically, these models yielded an R² value of 0.78 for RSAGB when compared against the calculated AGB (CAGB). Figure 17 illustrates the strong agreement between predicted and calculated AGB values reported in Table 7, confirming the robustness of satellite-based models in capturing biomass variability. This combined tabular and graphical analysis demonstrates the effectiveness of satellite-integrated models for accurate AGB estimation, particularly for reed grass within the plant population studied.
Model-1 and Model-2 were both derived using the same vegetation index; the two models differ in the allometric equation applied to convert the index value to AGB, which is why they achieve a similar R² while differing in absolute prediction error (see below). In addition to the individual spectral bands, including Red (R), Green (G), Blue (B), Near-Infrared (NIR), Red Edge (RE), and Deep Blue (DB), a set of vegetation spectral indices was used to characterize vegetation properties and assess their relationships with aboveground biomass. The vegetation indices included Chlorophyll Red Edge (ChL_RE), Green–Red Vegetation Index (GRVI), Normalized Difference Red Edge Index (NDRE), Normalized Difference Vegetation Index (NDVI), Red–Blue Ratio Index (RBRI), and Red Edge Simple Ratio/Red Edge Spectral Index (RE_SER). The Pleiades satellite image was acquired on 28 August 2023, while field destructive sampling commenced on 11 September 2023, corresponding to a 14-day interval between image acquisition and field sampling.
Table 7 also shows that Model-1 and Model-2 achieve nearly identical R² (0.781 vs. 0.783) despite a large difference in MAPE (7.90% vs. 27.80%). This is not contradictory: because both models are built from the same vegetation index but apply different allometric equations to convert that index into AGB, they capture the overall spatial trend in biomass equally well (hence the near-identical R²), while the two equations differ in their sensitivity to absolute prediction error, particularly on low-biomass plots. R² summarizes the proportion of variance explained across the full range of plots and is comparatively insensitive to a small number of large percentage errors, whereas MAPE is a percentage-based metric that is disproportionately inflated by poor absolute agreement on low-biomass plots, where even a small absolute error corresponds to a large relative error. We traced this discrepancy to the metric’s calculation basis: MAPE was computed in log(AGB) space, comparing predicted against actual ln(AGB) rather than the back-transformed AGB values. Because Model-2’s target values are systematically closer to zero than Model-1’s (a consequence of its more negative intercept), a modest absolute residual on plots with the lowest reed height produces a disproportionately large percentage error. Specifically, Plot 11 (2.2 m, the shortest reed height in the dataset) is the dominant contributor, with percent errors of up to 121% across its sampled points; Plot 8 is the second-largest contributor, with a consistent ≈68% error across its points. Excluding Plot 11 alone reduces Model-2’s MAPE from 27.8% to 18.9%. This behaviour is a known artifact of percentage-based error metrics when the reference value approaches zero, and does not indicate that Model-2 performs poorly on an absolute scale — its RMSE (0.065) and MAE (0.053) are, in fact, marginally better than Model-1’s.
Detailed maps illustrating the Remote Sensing Above Ground Biomass (RSAGB) for Reedgrass vegetation were constructed utilizing satellite imagery. These maps were instrumental in visualizing and depicting the distribution patterns of RSAGB across the Reedgrass plants. As depicted in Figure 18, the overlay of RSAGB information was superimposed onto the identified locations of the detected reed plants at a pixel-based resolution.
This overlaying technique facilitated a visual representation highlighting the relationship between RSAGB distribution and the specific spatial arrangement of detected reed plants within the satellite imagery. The resulting map provided a comprehensive insight into the correlation be- tween RSAGB patterns and the presence and distribution of reed plants, offering a detailed understanding of the biomass distribution dynamics across the Reed grass site.
In addition, intricate maps delineating carbon sequestration areas were meticulously crafted using satellite data in conjunction with Machine Learning algorithms (RS-Carbon-Seq.). These maps were specifically designed to visualize and analyze the distribution patterns of carbon sequestration areas derived from the RS-Carbon- Seq. methodology. As illustrated in Figure 19, an overlay technique was employed, showcasing the RS-Carbon-Seq. information superimposed onto the identified locations of detected Reed plants at a pixel-by-pixel resolution. This visual representation provided a comprehensive depiction of the relationship between the delineated areas of carbon sequestration as per RS-Carbon- Seq. and the specific spatial arrangement of identified Reed plants within the satellite imagery. This mapping approach facilitated a detailed exploration of the correlation between carbon sequestration zones and the distribution patterns of Reed plants, thereby contributing to an enhanced understanding of the interplay between carbon sequestration and the presence of Reed plants within the studied area.
3. Discussion
This study provides the first comprehensive, integrated assessment of biomass and carbon sequestration dynamics for Phragmites australis in a hyper-arid artificial wetland in Oman. By combining destructive sampling with remote sensing, we aimed to resolve the methodological challenges associated with carbon accounting in highly heterogeneous arid ecosystems.
The carbon stocks observed in this study, ranging from 0.36 to 1.95 kg/m² (equivalent to 3.6 to 19.5 Mg C/ha), demonstrate that P. australis maintains a substantial aboveground carbon pool even under extreme water stress. While intertidal blue carbon marshes are recognized for sequestering 1–2 Mg C per hectare per year [8], the total standing carbon stock observed at the Al Ansab wetland aligns with the higher end of global Phragmites productivity estimates. This confirms that artificial wetlands constructed for wastewater treatment in arid zones concurrently function as significant carbon sinks, adding a critical climate-mitigation dimension to their well-documented water purification services [11,12].
A pivotal finding of this research is that none of the simple field-measured biometric parameters tested — plant height, tiller density, fresh weight — showed a strong standalone correlation with destructively measured aboveground biomass (AGB) at this sample size. Height correlated only weakly with measured AGB (R² = 0.15), a magnitude comparable to the localized allometric models incorporating tiller density, fresh weight, and dry biomass (R² < 0.16); see Figure 12 and its caption for the distinction between this measured correlation and the near-perfect fit of the height-based allometric equations to their own input variable. This outcome is nonetheless informative for arid ecology. In temperate regions, tiller density is often a reliable predictor of biomass [14]; however, in hyper-arid environments, plants exhibit high phenotypic plasticity in response to micro-variations in water and salinity availability, and no single field-measured biometric variable captured this variability well enough to serve as a reliable standalone predictor. As evidenced by Plot 1 (214 thin tillers, moderate biomass) versus Plot 9 (73 robust tillers, high biomass), high tiller density does not equate to high carbon storage under arid stress, and height alone does not resolve this either. This is precisely why the remote-sensing approach, which integrates canopy-level spectral information rather than a single morphological measurement, is the more robust tool demonstrated in this study (R² = 0.78; Section 2.3): standard ground-based allometric equations developed in temperate or mesic environments [5] are likely inadequate for arid wetlands, and satellite-derived vegetation indices offer a more reliable path to biomass and carbon estimation than any single field-measured predictor tested here.
This correlation was re-examined in light of the small sample size (n = 12). Figure 12 plots, against reed height, both the destructively measured AGB values (Table 2) and the AGB values predicted by the two height-based allometric equations described in Section 2.2 (Model#1, from Conti et al. [2019]; Model#2, this study’s recalibration of that equation). These two series are not equally informative: because Model#1 and Model#2 compute AGB directly as a function of height, their predicted values are mathematically constrained to track height almost perfectly (R² = 0.999), independent of how well the underlying equation predicts real biomass — this reflects the equations’ internal consistency with their own input variable, not an independent validation. The scientifically meaningful test is the correlation between height and the destructively measured AGB values themselves, which is markedly weaker (R² = 0.15). We therefore revise our interpretation: height alone is not a strong standalone predictor of measured aboveground biomass in this dataset, and the R² value previously used to characterise this relationship should not be read as evidence that height predicts real biomass well.
The sample size of n = 12 destructive plots reflects the physical and ethical constraints of this study design: destructive sampling was restricted to preserve the integrity of the constructed wetland (an active wastewater-treatment facility), each plot required both oven-drying (105 °C, 48 h) and TOC analysis in triplicate batches, and accessibility within the reed oasis limited the number of locations that could be safely and non-disruptively sampled. This sample size limits the statistical power of the plot-level allometric models; we therefore present these models as a pilot-scale, hypothesis-generating result that should be validated with a larger and/or multi-season dataset before being applied predictively elsewhere.
The failure of traditional plot-level allometry in this study underscores the absolute necessity of remote sensing for carbon accounting in arid wetlands. Vegetation indices derived from satellite imagery achieved a high accuracy (R² = 0.78) in estimating spatial biomass variability, successfully overcoming the limitations of the ground-based allometric models. This aligns with global trends demonstrating the efficacy of optical remote sensing in wetland environments [28,32]. Remote sensing captures the spectral reflectance of the canopy, which is inherently linked to chlorophyll content, leaf area index, and vegetation structure—factors that collectively represent “plant vigor” better than simple physical counts. By averaging out the micro-scale heterogeneity (like the erratic tiller densities observed in our 12 plots), satellite-based models provide a spatially continuous and scalable estimation of biomass that destructive sampling alone cannot achieve [29,30].
Furthermore, the comparison between the Dry Weight Ratio and Total Organic Carbon (TOC) approaches revealed important methodological nuances. The TOC approach consistently yielded lower carbon stock estimates than the dry-weight ratio method. This is expected, as TOC analyzers specifically isolate oxidizable organic carbon, excluding inorganic carbonates that might be incidentally included in gross dry-weight mass calculations, particularly in alkaline arid soils. For future carbon credit methodologies (such as the UNFCCC’s Clean Development Mechanism), the TOC approach provides a more conservative, precise, and defensible metric for organic carbon sequestration.
From a management perspective, these findings hold profound implications for arid regions like Oman. Artificial wetlands, such as the Al Ansab site, are often established for waste management and biodiversity. However, this study demonstrates that with proper monitoring, these sites can be quantifiably valued as Nature-Based Solutions (NbS) for climate mitigation. Decision-makers must recognize that the ecosystem services provided by P. australis extend beyond local habitat provision to active atmospheric carbon removal. Moving forward, integrating field-inventory height data with satellite-derived vegetation indices offers a highly efficient, scalable framework for long-term carbon monitoring across the Gulf Cooperation Council (GCC) region’s expanding network of constructed wetlands.
4. Materials and Methods
Figure 20 summarises the overall workflow followed in this study. Data collection proceeded along two parallel but linked tracks. The first, ground-based track began with field plot layout and destructive sampling of 12 reed plots, followed by laboratory analysis of the harvested material to obtain dry weight and total organic carbon (TOC) content; these measurements were used to derive plot-level aboveground biomass (AGB) and carbon stock (Table 2) and to fit allometric regression models relating AGB to simple biometric predictors such as height, tiller density, and fresh weight. The second, remote-sensing track began with acquisition and pre-processing of Pleiades satellite imagery of the study site, followed by Support Vector Machine (SVM) classification to delineate reed cover and extraction of vegetation indices (VIs) from the classified imagery. The two tracks were then brought together in a final step that correlated the satellite-derived vegetation indices against the field-derived AGB and carbon-stock values, yielding the remote-sensing regression models (Model-1 and Model-2) evaluated in Section 2.3 and Table 7.
4.1. Experimental Design
The study of Phragmites australis, reed grass, wetland was carried out in Al Ansab wetland located 15 kilometers from the heart of Muscat the Capital of the Sultanate of Oman, at the precise coordinates of 23◦ 33’ 46.4076” N, 58◦ 20’1.86” E (Figure 21 and Figure 22). Originally constructed on a smaller scale, the site was expanded towards the north-east by the addition of a buffer zone on July 7th, 2008. Nowadays, the wetland encompasses a total land area of approximately 40 hectares (ha), which includes a lagoon and a range of associated habitats. As a man-made wet- land, it is distinct from natural wetlands but still serves an important ecological function in providing a habitat for a variety of flora and fauna. The wetland processes and treats sewage effluent, resulting in clear water. The wetland is therefore a crucial site for ecological research and environmental conservation efforts in the region. A stratified random sampling approach was utilized to assess the aboveground biomass of Phragmites australis. This methodology falls under the category of destructive techniques and is aligned with the Clean Development Mechanism (CDM) method- ologies overseen by the United Nations Framework Convention on Climate Change (UN-FCCC).
The research site was subjected to thorough surveys using a random approach to gather data from plants for destructive sampling purposes. A total of 12 plots of Phragmites australis, measuring 1 meter by 1 meter were sampled. The collected data included counting the number of reeds per plot, their height, fresh weight, and coordinates. The precise locations of each plot were determined using a Global Positioning System (GPS) in combination with local mapping stations, guaranteeing an accuracy level of 0.1m. This was done to mark the position of the sampling plot within the reed wetlands, ensuring accurate positioning of the randomly selected plots.
4.2. Sample Processing and Laboratory Measurements
Figure 23 delineates the systematic procedure of the destructive sampling technique for the designated plots. The destructive sampling commenced with preliminary measurements in step 1. The diagram navigates through subsequent stages until step 6, where freshly gathered reed samples are transported to the laboratory for dedication. The sequence initiates with the identification and measurement of reed plots for destructive sampling, followed by the implementation of the destructive procedure. The total weight of fresh reeds is then ascertained using a caliper, and sub- samples are weighed, labeled, and dispatched to the laboratory for desiccation. Additionally, the height of the reeds and the number of stands per plot are measured. This visual representation offers a structured overview of the sampling process, ensuring precise data collection for a thorough analysis of carbon sequestration and associated variables.
The field data collection and measurements were carried out in three distinct phases:
Measurement of key biometric variables in standing reeds: This involved measuring total height (m) and number of reeds per 1 m2.
Determination of fresh biomass: The stems of Phragmites australis were severed at ground level and subsequently tallied. After harvesting the 12 plots of reeds, the fresh above-ground biomass weight was measured.
Collection of samples for dry biomass de-- termination: two samples of the mixture of each reeds plot (ranging from 200 to 500 g) were collected to estimate its carbon content and dry process. These samples were prepared directly on site and passed to the university lab on the same day to be dried in an oven at 60◦-80C◦ until a constant weight was achieved [13]. The samples were stored in sealed plastic bags and weighed on the same day of cutting using a Pitney Bowes scale (capacity: 0–2.5 kg). The 2nd samples were carried out to get the total organic carbon content (TOC) method to estimate biomass by determining the amount of organic carbon present in the plant material. Carbon compounds were first extracted from 0.5–1 g of each reed’s dried plot sample using a mixed-acid digestion method (0.0125 M H2SO4 and 0.05 M HCl); the resulting digested extract was then analyzed for organic carbon content using a TOC-V Analyzer via elemental analysis/combustion.
The procedure for assessing dry biomass adhered to established protocols detailed in the SOP Wood Density [33] and SOP Destructive sampling [34]. However, this study employed two dis- tinct methods to estimate the carbon sequestration of Phragmites australis (Reed grass): one involved dry sampling biomass steps, while the other utilized the laboratory total organic carbon concentration method. In this context, reeds were classified as non-woody plants for these assessments.
A total of 12 plots containing Phragmites australis specimens were evaluated, with samples meticulously stored in plastic bags to ensure their integrity and prevent moisture loss. These samples were subsequently transported to the Sultan Qaboos University (SQU) laboratory for further analysis using both methods. To estimate the biomass of the reed plots, full-weight calculations and sub-samples were utilized. Each of the 12 plot samples was taken to the lab’s drying room, where they were dried and weighed to determine the dry weight of the entire plots. This methodology, in accordance with IPCC Methodological Guidelines (IPCC, 2014) [35], involved the systematic randomization of sampling plots for Phragmites australis across accessible zones. This randomization process utilized GPS coordinates obtained with an LT700H 8” Android RTK Tablet and GNSS Antenna AT312.
Upon arrival at the laboratory, samples were weighed to determine fresh weight. Following initial weighing, samples underwent air-drying in paper bags to remove excess moisture before being oven-dried at 60◦C, following [34] and IPCC, 2014 methodology. Daily weighing during drying deter- mined stable dry weight, allowing calculation of the percentage of dry weight relative to original fresh weight using the dry-to-fresh factor (DF), facilitating the determination of the ratio between dry weight and original fresh weight for each sample.
where SDW is sample dry weight (kg),and SWW is sample wet weight (kg).
Furthermore, the equation of [36] of non woody plants could be used to calculate the dry biomass of the reeds:
where , ADWR is average dry to wet ratio, FPW is full plot weight (kg), ODW is Total oven dry weight , TFW is Total fresh weight (kg), SFW = Sample fresh weight (kg), and SODW = Sample oven dry weight (kg).
On the other hands, Total Organic Carbon (TOC) method: The TOC method estimates biomass by determining the amount of organic carbon present in the plant material. This method involves collecting plant samples, drying them to remove moisture, and then analyzing the carbon content using laboratory techniques such as elemental analysis or combustion. The concentrations of Total Organic Carbon (TOC) in the reedgrass samples were quantified using a TOC analyzer, a widely recognized and reliable instrument for determining carbon content. The TOC method pro- vides an indirect estimation of biomass based on the assumption that a certain proportion of the plant’s organic carbon is derived from biomass. The actual proportion can vary depending on the plant species and environmental factors, so it is essential to calibrate the method for specific ecosystems.
The carbon stock in the reedgrass samples was subsequently calculated based on the TOC con- centration, expressed as a percentage, multiplied by the corresponding dry weight of the sample. The resulting carbon stock values were then ex- pressed in grams per square meter (g/m2), pro- viding a quantitative measure of the carbon con- tent within the reedgrass ecosystem. By employing this rigorous methodology, encompassing sample collection, preparation, analysis, and calculation, a comprehensive evaluation of the carbon stock in the reedgrass samples was accomplished, allowing for a more profound understanding of the carbon dynamics within the studied ecosystem.
The allometric relationship between plant height and aboveground biomass (AGB) was modeled using a power function of the form:
AGB = a × Hb
where AGB represents aboveground biomass (kg/m²), H is plant height (m), and a and b are regression coefficients determined empirically.
In addition, carbon stock (C) was estimated using:
C = AGB × CF
where CF represents the carbon fraction derived either from dry biomass or measured Total Organic Carbon (TOC) content.
4.3. Above Ground Biomass and Carbon Sequestration
A specified number of individual plots of Phragmites australis (reed grass) were selected from the targeted area to measure various parameters such as reed height (H), the number of reed stems per plot, and the total fresh weight per plot. Reed height measurements were conducted using an Electronic Clinometer. Subsequently, all selected reed plots were harvested to determine their respective fresh weights, which constituted the total Aboveground Biomass (AGB). In the field, fresh samples were weighed, well-mixed, and subsamples were placed in marked bags. The subsample was then utilized to establish an oven dry to wet mass ratio, which was subsequently used to convert the total wet mass to oven dry mass. A subsample was taken to the laboratory and oven-dried until a constant weight was achieved following the methods outlined by [36,37].
The initial approach involved the use of the dry- to-fresh ratio method, which calculates biomass
by considering the weight ratio of dried reed samples to their corresponding fresh weight. The second method, known as the Total Organic Carbon (TOC) method, estimates Aboveground Biomass (AGB) by measuring the total organic carbon content of reed samples. Alongside these methods, insights from [38], study on similar plant species were incorporated. Conti research [38] provided a valuable benchmark for evaluating the performance of the dry-to-fresh ratio and TOC methods when applied to reeds.
A regression equation (equation 6) was utilized to estimate AGB using variables such as weight (H and CD), where AGB represents the total aboveground biomass of individual reed plots measured in 1m*1m and expressed in kilograms (kg). Here, CD refers to the canopy diameter of the plot in meters (m), and H represents the height of the reeds in meters (m), with ’e’ symbolizing the natural logarithm (LN) constant. The regression analysis employed four distinct models sourced from relevant studies to conduct a comparative assessment based on their correlation indicators like R2 values and correlations with reed indicators such as height, diameter, and canopy. This evaluation aimed to determine the fitting ac- curacy of the models concerning the actual measured destructive aboveground biomass, as elaborated in equation 6.
where, H: height of reeds (m), and D: plot canopy diameter CD (m2)
Through a meticulous examination of both the dry-to-fresh ratio and TOC methods, along with insights gleaned from Conti et al.’s (2019) study, the researchers sought to gain a comprehensive understanding of the most effective and accurate approach for estimating the aboveground biomass of reeds. By comparing these methodologies, this study aimed to contribute valuable insights to the field of wetland vegetation biomass estimation and advance knowledge in ecological modelling.
The calculation of aboveground reed biomass encompassed evaluating the total weights of the reeds above the harvested ground. It is worth not- ing that all plant tissues typically contain between 45-50% carbon, making this estimation suitable for various samples, including dead and live samples [34]. At a global scale, carbon contents in plant organs vary, ranging from 45.0% in reproductive organs to 47.9% in stems, particularly in the woody parts (Suhui et al., 2018). Al- though there is no universally accepted conversion value for biomass to carbon content, the IPCC 2006 suggests a range of 45% to 50%, which is commonly adopted as the default value for many trees. The assessment of the carbon storage capacity of plants involved integrating biomass values with a carbon default value or carbon factor (CF) typically below 0.50 [39,40]. For converting the carbon content into CO2 equivalent (CO2eq), the carbon quantity was multiplied by 3.67, reflecting the ratio of the molecular weight of car- bon dioxide to the atomic weight of carbon [41].
The determination of total carbon storage in vegetation involves the multiplication of vegetation biomass, the carbon conversion factor, and the area under consideration [42]. The carbon conversion factor denotes the proportion of carbon content within the vegetation and exhibits variability across different vegetation types [42]. For the purpose of this study, the carbon storage assessment focused exclusively on the predominant vegetation of the estuary salt marsh communities, namely Phragmites australis, which possesses a carbon conversion factor of approximately 0.50, consistent with the value applied throughout this study. It is important to note that this specific value applies solely to Phragmites australis. The estimation of carbon storage values was conducted as follows:
where, Cplant is the carbon storage in the Phragmites community (g), SB is the above ground standing biomass of Phragmites (g m2), and Aplant is the area occupied by the Phragmites community (m2).
Table 4 Summarizes the carbon stock measurements conducted on Phragmites australis plants. Across the 12 sampled plots in this study, the dry-weight ratio approach yielded an average AGB of 2.22 kg/m² and a corresponding average carbon stock of 1.11 kg/m² (applying the 0.50 carbon conversion factor, Table 2). The TOC analyzer approach, which measures carbon content directly rather than deriving it from AGB, gave an average carbon stock of 0.79 kg/m² (mean TOC content of 17.3%, Table 2). [43] examined dry samples and reported an AGB of 1.853 kg/m2, with a carbon content of 0.81 kg/m2, specifically representing 80% of the below-ground biomass (BGB) in the range of 3.3 - 1.46 kg/m2. [44] investigated the carbon stock in Pristine Salt Marsh and found a range of 0.642 kg/m2 to 3.0-35.6 kg/m2. Additionally, impacted salt marshes exhibited carbon stock densities ranging from 1.04 kg/m2 to 8.6-24.0 kg/m2. [45] observed a wide range of carbon stock densities, varying from 0.31-52.90 Mg/ha (mean: 0.733 kg/m2).
Reported above-ground biomass (AGB) and carbon content measurements exhibit significant variation across different methods and locations, ranging from 1.6 to 62.3 kg/m2. In this study, average AGB was estimated at 2.22 kg/m² using the dry-weight ratio approach, with a corresponding average carbon stock of 1.11 kg/m² (dry-ratio) and 0.79 kg/m² (TOC approach). Comparatively, other studies reported AGB values such as 1.853 kg/m2 from dry samples, 0.642 kg/m2 in pristine salt marshes, and 1.04 kg/m2 in impacted salt marshes. Larger- scale estimates include Egypt with 30.4 MT ha-1 year-1 (3.04 kg/m2), Iraq with 13.6 MT ha-1 year-1 (1.36 kg/m2), Minnesota with 16.8 MT ha-1 year-1 (1.68 kg/m2), and Sweden with values ranging from 9.9 to 25.1 MT ha-1 year-1 (0.99–2.51 kg/m2). These variations highlight the influence of environmental conditions and methodological differences on biomass and carbon stock estimations.
Overall, the table highlights the variability in carbon stock measurements in Phragmites australis plants across different locations and methodologies. These findings contribute to our understanding of the carbon dynamics in this plant species and its implications for carbon sequestration and ecosystem carbon storage.
Reed carbon stocks stograe (CSS), kg, were appraised through the conversion of the computed destructive biomass of the reed plots, employing a standard factor of 0.50 as applied throughout this study, assuming the reeds as non-woody plants [42]. Moreover, for determining the CO2 equivalent (CO2eq), the amount of carbon was multiplied by 3.67, representing the ratio between the molecular weight of carbon dioxide and the atomic weight of carbon [41].
where CSS is Carbon stock storage (kg), and TDR is Reed dry biomass (kg).
where 0.001 = factor for converting CO2eq from kg to tone.
4.4. Sampling and Analytical Method – Statistical Analyses
The process employed to construct Allometric models for Above Ground Biomass (AGB) in- volved regression analysis, where the aboveground biomass was regressed against independent variables such as reed height (H), canopy diameter (CD), and the number of reed stems per plot, with Ln (AGB) serving as the dependent variable. Two approaches for calculating AGB were considered: one derived from dry biomass (Dry Ratio AGB) and the other from Total Organic Carbon (TOCAGB), both correlated as dependent variables with the independent variables of the reed plots.
Initially, the correlation between the actual AGB obtained through destructive methods and the tested generalized allometric equations, outlined in equation 6 [38], was examined using Minitab software for data analysis. Separate log-log models were fitted for each individual allometric variable to identify the most effective predictor for AGB. The evaluation of these log-log models incorporated crucial metrics such as R2 and P-Value.
where H is height of reeds (m), and D is the plot canopy diameter (CD) (m2).
Statistical analyses were conducted to evaluate the relationships between measured plant variables and biomass estimates. Regression models (linear and nonlinear) were developed to assess the predictive performance of selected variables, particularly plant height, in estimating aboveground biomass (AGB). Model performance was evaluated using standard statistical indicators, including the coefficient of determination (R²), mean absolute error (MAE), and root mean square error (RMSE). This assessment focused exclusively on the fit- ting dataset to assess the performance of local models and compare them against previously established models. The biomass of each reed was then calculated using the previously tested equations and the most suitable equation developed in this study. A comparison was carried out using an ANOVA test.
4.5. Testing Established Allometric Model Equation
In this investigation, the biomass estimated at the plot scale using the allometric equation was referred to as the observed biomass. The study conducted by [38] served as the fundamental basis for our research in formulating the allometric equations, along with relevant studies focusing on similar plant species. Conti’s study extensively analyzed and assessed prior research concerning actual destructive plants, accounting for errors and limitations. Their protocol was recommended for applying general above-ground biomass (AGB) models and involved the development of allometric equations for predicting individual above- ground biomass.
Consequently, datasets from destructively sampled reed biomass were compared to assessing their correlation indicators, specifically R2 values, with the tested equations in area-based biomass assessment. The assessment of Phragmites australis (reed grass) involved 12 destructive plots, showcasing linear relationships with high R2 values for most of the assessed equations.
4.6. Developing a Local Remote Sensing Model
The estimation of Above Ground Biomass (AGB) in the Phragmites australis (reed grass) area of interest was conducted using both the destructive method, TOC method along with re- mote sensing method. Pleiades sensor satellite im- ages was used in this approach, which were obtained prior to the destructive sampling of plants. The acquisition date for these images was August 28, 2023, and the image had a resolution of 30cm with seven spectral bands: deep blue, blue, green, red, near-infrared, and panchromatic. High-resolution ortho mosaics were used to compute various vegetation indices (VIs), and corresponding raster layers were created based on these indices.
To minimize interference stemming from soil, roads, water bodies, and weeds within the raster layers, binary masks were created using orthorectified images and the Support Vector Machine (SVM) as a classifier. Zonal statistics techniques were subsequently employed to ascertain the aver- age pixel values at each sampling location across these raster layers, establishing correlations with ground-based biomass measurements. To streamline and standardize these procedures, ArcGISPro and a machine learning-driven programming language were utilized to automate the extraction of Vegetation Indices (VIs) and the removal of soil/weed interference.
Various vegetation indices (VIs) were computed using data from Near-Infrared to Red (NIR-R), Near-Infrared to Red-Edge (NIR-RE), and Spectrometer sources. The recommended VIs (outlined in Table 8) in this study was formulated using digital numbers (DNs) derived from red, green, and blue bands (RGB) within the captured images. These proposed VIs were employed to evaluate band characteristics related to biophysical properties such as leaf greenness and chlorophyll content. Additionally, adjustments were made to the inherent factors of specific VIs, such as the correction factor in the Soil-Adjusted Vegetation Index (SAVI).
Remote sensing data were integrated to evaluate the potential for large-scale biomass estimation. Spectral information was used to calculate vegetation indices, including normalized difference vegetation index (NDVI), soil-adjusted vegetation index (SAVI), and near-infrared-based indices (e.g., NIR-R and NIR-RE). These indices were correlated with field-measured biomass data to assess their effectiveness in predicting spatial variability in aboveground biomass. The approach enables extrapolation of plot-level measurements to broader spatial scales. A sequence of commonly utilized vegetation indices (VIs) was computed using high-resolution ortho mosaics, generating corresponding raster layers (Table 8). Binary masks were then created based on orthorectified images to remove interference from soil, roads, water, and weeds, employing Sup- port Vector Machine (SVM) as a classifier. Zonal statistics were subsequently applied to determine average pixel values across these layers at each sampling location, establishing associations with ground-based biomass measurements.
To streamline and standardize the processes, the ArcGIS library and programming language were utilized for automating VI extraction and eliminating soil/weed interference. The process of plant delineation through spectral analysis indices and composite layers commenced with investigating all single and combined vegetation indices, selecting the most suitable indices based on available satellite image sensor bands (R, G, B, Near Infrared, Red Edge, and Deep Blue). Following this, indices were stacked to construct a composite layer using the composite command from ArcGIS software modeling. A supervised classification was then conducted on the composite images using the support vector machine method, incorporating field measurements to delineate targeted plants in the classification process.
Detailed classifier parameters (kernel type) and formal accuracy metrics (overall accuracy, Kappa coefficient) for this classification step were not recorded during the original analysis and could not be reconstructed for this revision; this is acknowledged as a limitation of the remote-sensing workflow, and we recommend that future work incorporate a formal accuracy assessment (e.g., a confusion matrix with held-out validation samples) to support reproducibility.
Additionally, a classification map was generated to depict various classes such as soil, roads, buildings, crops, and delineated plants in separate categories. Subsequently, the class representing delineated plants was selected from the classification map and exported as a feature class, which would be used for AGB estimation correlation modeling.
Remote sensing techniques were utilized for data collection regarding plant biomass and canopy area index, serving as input for machine learning algorithms dedicated to estimating the carbon sequestration capacity of these plants. Concurrently, Geographic Information Systems (GIS) played a pivotal role in integrating spatial data, enabling the creation of precise maps delineating the study area.
The methodology and analysis steps under- taken in this research are illustrated in Figure 24, showcasing a process involving a destructive method. This method entails gathering plant material to acquire essential data for estimating the carbon stock within the plants. The destructive approach involves collecting samples of plant tis- sue for subsequent laboratory analysis, including techniques like carbon analysis. The data obtained through the destructive method were then compared and correlated with information gathered through remote sensing and GIS.
5. Conclusions
Similarly, in hyper-arid artificial wetlands, accurate assessment of ecosystem services such as carbon sequestration requires methods adapted to stress-driven plant variability. While Phragmites australis maintains significant carbon stocks, conventional allometric models fail under conditions of morphological plasticity. In contrast, satellite-derived vegetation indices — rather than field-measured height alone, which correlated only weakly with destructively measured biomass in this dataset — provide a robust and scalable framework for carbon monitoring. Overall, these findings demonstrate that successful management of arid systems—whether addressing contaminant risks in agriculture or quantifying blue carbon in wetlands—depends on leveraging species-specific physiological traits alongside targeted monitoring approaches.
Author Contributions
Conceptualization & methodology, K.J. and Y.A.; writing—original draft preparation, K.J. and Y.A.; writing—review and editing, K.J, Y.A, M,S, H.S, A.T, and A.B. All authors have read and agreed to the published version of the manuscript.
Funding
This research work was funded by The Petroleum Development Oman as well as logistics support and in-kind contributions by SQU under a grant code number of CR/DVC/GISC/22/03.
Data Availability Statement
The data presented in this study is available on request from the corresponding author.
Acknowledgments
The authors thank B.K Al-Jabri, Y.K Al-Jabri, A.E Al-Muqbali, Z.A Al-Jardani, M.Y Al-Wahidi, D.Al-shihi, M.I. Al- Belushi, A.A. Basra, and T.M Al-Jabri for their support during the experiment.
Conflicts of Interest
The authors have no relevant financial or non-financial interests to disclose.
Abbreviations
The following abbreviations are used in this manuscript:
| AGB | Aboveground Biomass | H | Reed Height |
| BGB | Average Dry to Wet Ratio | RSAGB | Remote Sensing Aboveground Biomass |
| BGB | Below-Ground Biomass ( | RMSE | Root Mean Square Error |
| BAF | Bioaccumulation Factors | SDW | Sample Dry Weight |
| CD | Canopy Diameter | SODW | Sample Oven Dry Weight |
| C | Carbon | SWW | Sample Wet Weight |
| CSS | Carbon Stock Storage | SAVI | Soil-Adjusted Vegetation Index |
| CDM | Clean Development Mechanism | SQU | Sultan Qaboos University |
| GPS | Global Positioning System | SAR | Synthetic Aperture Radar |
| LiDAR | Light Detection and Ranging | TFW | Total Fresh Weight |
| MAE | Mean Absolute Error | TOC | Total Organic Carbon |
| MAPE | Mean Absolute Percentage Error | TOCAGB | Total Organic Carbon Aboveground Biomass |
| Ln | Natural Logarithm | TF | Translocation Factor |
| NIR-RE | Near-Infrared to Red-Edge | TDR | Tree Dry Biomass |
| NIR-R | NIR to Red Ratio | VIs | Vegetation Indices |
| ODW | Oven Dry Weight |
References
- C. J. Anderson, D. Heins, K. C. Pelletier, J. L. Bohnen, J. F. Knight, Mapping invasive Phragmites australis using unoccupied aircraft system imagery, canopy height models, and synthetic aperture radar, Remote Sensing 13 (16) (2021).
- P. J. Hocking, C. M. Finlayson, A. J. Chick, The biology of Australian weeds. 12. Phragmites Aus- tralis(Cav.) Trin. ex Steud, Journal of the Australian Institute of Agricultural Science 49 (3) (1983) 123– 132.
- S. M. Galatowitsch, N. O. Anderson, P. D. Ascher, Invasiveness in wetland plants in temperate, North America. Wetlands 19 (1999) 733–755.
- R. M. Chambers, D. T. Osgood, D. J. Bart, F. Mon- talto (2003).
- Y. Du, J. Wang, Y. Lin, Z. Liu, H. Yu, H. Yi, Esti- mating the Aboveground Biomass of Phragmites Aus- tralis (Common Reed) Based on Multi-Source Data, IGARSS 2018-2018 IEEE International Geoscience and Remote Sensing Symposium (2018) 9241–9244.
- E. Mcleod, G. L. Chmura, S. Bouillon, R. Salm, M. Björk, C. M. Duarte, . . Silliman, B. R, A blueprint for blue carbon: toward an improved understanding of the role of vegetated coastal habitats in sequester- ing CO2, Frontiers in Ecology and the Environment 9 (10) (2011) 552–560.
- K. B. Byrd, L. Ballanti, N. Thomas, D. Nguyen, J. R. Holmquist, M. Simard, L. Windham-Myers, A remote sensing-based model of tidal marsh aboveground car- bon stocks for the conterminous United States, IS- PRS Journal of Photogrammetry and Remote Sens- ing 139 (2018) 255–271.
- L. Pendleton, D. C. Donato, B. C. Murray, S. Crooks, W. A. Jenkins, S. Sifleet, . . Baldera, A (2012).
- S. D. Bridgham, J. P. Megonigal, J. K. Keller, N. B. Bliss, C. Trettin, The carbon balance of North Amer- ican wetlands, Wetlands 26 (4) (2006) 889–916.
- C. M. Duarte, J. J. Middelburg, N. Caraco, Major role of marine vegetation on the oceanic carbon cycle, Biogeosciences 2 (1) (2005) 1–8.
- D. A. White, J. M. Visser, Water quality change in the Mississippi River, including a warming river, explains decades of wetland plant biomass change within its Balize delta, Aquatic botany 132 (2016) 5–11.
- B. Oteman, A. Scrieciu, T. J. Bouma, A. Stanica, D. V. D. Wal, Indicators of expansion and retreat of Phragmites based on optical and radar satellite remote sensing: a case study on the Danube delta, Wetlands (6) (2021) 41–41.
- K. Soetaert, M. Hoffmann, P. Meire, M. Starink, D. V. Oevelen, S. V. Regenmortel, T. Cox, Mod- eling growth and carbon allocation in two reed beds (Phragmites australis) in the Scheldt estuary, Aquatic Botany 79 (3) (2004) 211–234.
- R. Wan, P. Wang, X. Wang, X. Yao, X. Dai, Mapping aboveground biomass of four typical vegetation types in the Poyang Lake wetlands based on random for- est modelling and landsat images, Frontiers in Plant Science 10 (2019).
- X. Dai, G. Yang, D. Liu, R. Wan, Vegetation car- bon sequestration mapping in herbaceous wetlands by using a MODIS EVI time-series data set: a case in Poyang lake wetland, China. Remote Sensing 12 (18) (2020).
- C. L. Doughty, J. A. Langley, W. S. Walker, I. C. Feller, R. Schaub, S. K. Chapman, Mangrove range expansion rapidly increases coastal wetland carbon storage, Estuaries and Coasts 39 (2016) 385–396.
- M. Simard, L. Fatoyinbo, C. Smetanka, V. H. Rivera- Monroy, E. Castañeda-Moya, N. Thomas, T. V. D. Stocken, Mangrove canopy height globally related to precipitation, temperature and cyclone frequency, Nature Geoscience 12 (1) (2019) 40–45.
- T. J. Arkebauer, J. P. Chanton, S. B. Verma, Kim, Field measurements of internal pressurization in Phragmites australis(Poaceae) and implications for regulation of methane emissions in a mid- latitude prairie wetland, American Journal of Botany 88 (4) (2001) 653–658.
- S. R. Wolfer, E. H. V. Nes, D. Straile, Modelling the clonal growth of the rhizomatous macrophyte Pota- mogeton perfoliatus, Ecological modelling 192 (1-2) (2006) 67–82.
- T. Asaeda, S. Karunaratne, Dynamic modeling of the growth of Phragmites australis: model description, Aquatic Botany 67 (4) (2000) 301–318.
- Y. Yi, H. Xie, Y. Yang, Y. Zhou, Z. Yang, Suitable habitat mathematical model of common reed (Phrag- mites Australis) in shallow lakes with coupling cellu- lar automaton and modified logistic function, Ecolog- ical modelling 419 (2020).
- E. M. Eid, K. H. Shaltout, Y. M. Al-Sodany, Soetaert, K. Jensen, Modeling growth, carbon al- location and nutrient budgets of Phragmites Austral- isin Lake Burullus, Egypt. Wetlands 30 (2010) 240– 251.
- S. Zheng, D. Shao, T. Asaeda, T. Sun, S. Luo, M. Cheng, Modeling the growth dynamics of Spartina alterniflora and the effects of its control measures, Ecological Engineering 97 (2016) 144–156.
- T. Asaeda, D. N. Hai, J. Manatunge, D. Williams, J. Roberts, Latitudinal characteristics of below-and above-ground biomass of Typha: a modelling ap- proach, Annals of Botany 96 (2) (2005) 299–312.
- T. Asaeda, P. Sharma, L. Rajapakse, Seasonal pat- terns of carbohydrate translocation and synthesis of structural carbon components in Typha angustifolia, Hydrobiologia 607 (2008) 87–101.
- K. Al-Jabri, Y. Al-Mulla, F. Melgani, A. Stefanakis, Remote Sensing Analysis for Vegetation Assessment of a Large-Scale Constructed Wetland Treating Pro- duced Water Polluted with Oil Hydrocarbons, Re- mote Sensing 15 (24) (2023).
- Hammer, D. A. (Ed.). (Eds.), Constructed wetlands for wastewater treatment: municipal, industrial and agricultural, CRC Press, 1989.
- S. Wang, S. Li, S. Zheng, W. Gao, Y. Zhang, B. Cao, Shao, D, Estimating biomass and carbon seques- tration capacity of Phragmites australis using remote sensing and growth dynamics modeling: A case study in Beijing hanshiqiao wetland nature reserve, China. Sensors 22 (9) (2022) 3141–3141.
- K. B. Byrd, J. L. O'connell, S. D. Tommaso, M. Kelly (2014).
- Mutanga, E. Adam, M. A. Cho, High den- sity biomass estimation for wetland vegetation using WorldView-2 imagery and random forest regression algorithm, International Journal of Applied Earth Observation and Geoinformation 18 (2012) 399–406.
- Aslan, A. F. Rahman, M. W. Warren, S. M. Robe- son (2016).
- S. Luo, C. Wang, X. Xi, F. Pan, M. Qian, D. Peng, . . Lin, Y, Retrieving aboveground biomass of wetland Phragmites australis(common reed) using a combi- nation of airborne discrete-return LiDAR and hyper- spectral data, International journal of applied earth observation and geoinformation 58 (2017) 107–117.
- G. Reyes, Wood densities of tropical tree species, Vol. 88, Forest Service, Southern Forest Experiment Station, 1992.
- K. Goslee, S. M. Walker, A. Grais, L. Murray, Casarim, S. Brown (2016).
- B. F. Clough, P. Dixon, O. Dalhaus, Allometric re- lationships for estimating biomass in multi-stemmed mangrove trees, Australian Journal of Botany 45 (6) (1997) 1023–1031.
- V. Sharma, H. Chand, N. Rai, M. Prasad (2017).
- R. D. Lasco, F. B. Pukhil, V. O. C. R, J. M. Pulhin, S. S. N. Roy (2005).
- G. Conti, L. D. Gorne, S. R. Zeballos, M. L. Lipoma, Gatica, E. Kowaljow, . . Fernandes, P. M, Develop- ing allometric models to predict the individual above- ground biomass of shrubs worldwide, Global Ecology and Biogeography 28 (7) (2019) 961–975.
- M. Mngadi, J. Odindi, O. Mutanga (2021). URL . [CrossRef]
- G. Shen, Z. Wang, C. Liu, Y. Han (2020). URL . [CrossRef]
- Amiri, J. Ottelin, J. Sorvari, S. Junnila, Cities as Carbon Sinks-Classification of Wooden Buildings, Environmental Research Letters 15 (2020).
- Howard, Hoyt, Isensee, Telszewski, Pidgeon, Howard, J., Hoyt, S., Isensee, K., Telszewski, M., & Pidgeon, E. (2014). Coastal blue carbon: methods for assessing carbon stocks and emissions factors in mangroves, tidal salt marshes, and seagrasses. (2014).
- Dong, Dong, W., Shu, J., He, P., Ma, G., & Dong, M. (2012). Study on the carbon storage and fixation of phramites autralis in Baiyangdian demonstration area. Procedia Environmental Sciences, 13, 324-330. (2012).
- Byun, Lee, S. H, Kang, Byun, C., Lee, S. H., & Kang,H. (2019). Estimation of carbon storage in coastal wetlands and comparison of different management schemes in South Korea. Journal of Ecology and Environment, 43(1), 1-12. (2019).
- CHEN, Ji, et al. Depth-dependent responses of soil organic carbon stock under annual and perennial cropping systems. Proceedings of the National Academy of Sciences, 2022, 119.28: e2203486119.
- El-Kady, El-Kady, H. (2000). Seasonal variation in phytomass and nutrient status of Phragmites aus- tralis along the water courses in the middle Nile Delta, Egypt. Taeckholmia, 20(2), 123-138. (2000).
- Rezk, Al-Edany, Rezk, M. R. and Al-Edany, T. Y. 1980. Ecology of Phragmites austeralis (Cov.) Trin ex Steud. In Shatt Al-Arab, IRAQ. Part 1. seasonal and regional variations in the chemical constituents of water and soil in reed bebs. Pol. Arch. Hydrobiol. 27(3) : 349- 358. (1980).
- Pratt, Dubbe, Garver, Linton, Pratt, D. C., Dubbe,D. R., Garver, E. G., & Linton, P. J. (1984). Wetland Biomass Production: emergent aquatic management options and evaluations. A final subcontract report.[Includes a bibliography containing 686 references on Typha from biological abstracts] (No. SERI/STR-231-2383). Minnesota Univ., St. Paul (USA). (1984).
- Granéli, Granéli, W. (1984). Reed Phragmites australis (Cav.) Trin. ex Steudel as an energy source in Sweden. Biomass, 4(3), 183-208. (1984).
- S. Ahmad, J. F. Reid, Evaluation of colour repre- sentations for maize images, Journal of Agricultural Engineering Research 63 (3) (1996) 185–195.
- M. Louhaichi, M. M. Borman, D. E. Johnson, Spa- tially located platform and aerial photography for documentation of grazing impacts on wheat, Geo- carto International 16 (1) (2001) 65–70.
- GITELSON, Anatoly A., et al. Novel algorithms for remote estimation of vegetation fraction. Remote sensing of Environment, 2002, 80.1: 76-87.
- T. Hague, N. D. Tillett, H. Wheeler, Automated crop and weed monitoring in widely spaced cereals, Preci- sion Agriculture 7 (2006) 21–32.
- E. M. Barnes, T. R. Clarke, S. E. Richards, P. D. Colaizzi, J. Haberland, M. Kostrzewski, . . Moran, M. S, Coincident detection of crop water stress, ni- trogen status and canopy density using ground based multispectral data, in: Proceedings of the fifth in- ternational conference on precision agriculture, Vol. 1619, 2000.
- W. Rouse, R. H. Haas, D. W. Deering, J. A. Schell, J. C. Harlan (1974).
- C. F. Jordan, Derivation of leaf-area index from qual- ity of light on the forest floor, Ecology 50 (4) (1969) 663–666.
- B. T. W. Putra, P. Soni, Evaluating NIR-Red and NIR-Red edge external filters with digital cameras for assessing vegetation indices under different illu- mination, Infrared Physics & Technology 81 (2017) 148–156.
- Z. Zhen, S. Chen, W. Qin, J. Li, M. Mike, B. Yang, A modified transformed soil adjusted vegetation indexfor cropland in Jilin Province, China. Acta Geologica Sinica-English Edition 93 (S3) (2019) 173–176.
Figure 1.
Destructive sampling of Phragmites australis (Reed grass), a: site location of targeted plants, b-f cutting process of grass targeted plots (~ 1m * 1m), g: collection of fresh weight on site, h: collecting samples of 12 plots for lab drying process and samples in drying room.
Figure 1.
Destructive sampling of Phragmites australis (Reed grass), a: site location of targeted plants, b-f cutting process of grass targeted plots (~ 1m * 1m), g: collection of fresh weight on site, h: collecting samples of 12 plots for lab drying process and samples in drying room.
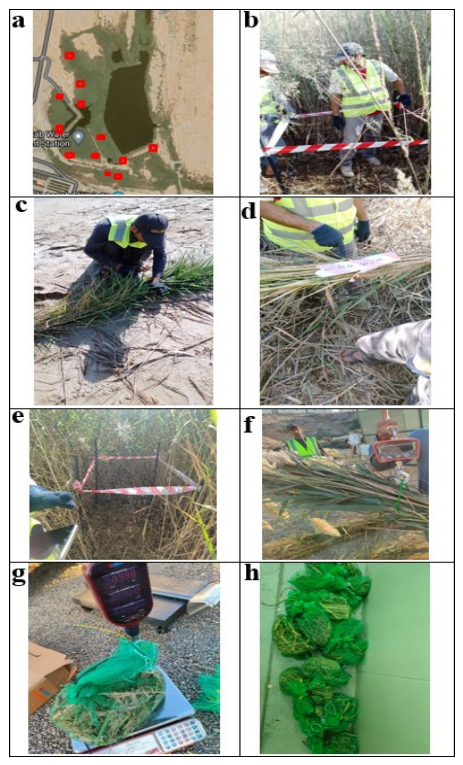
Figure 2.
TOC of Phragmites australis (Reed grass) Destructive sampling, a-f: TOC calculation of 12 plots samples in 3 batches using TOC-V Analyzer.
Figure 2.
TOC of Phragmites australis (Reed grass) Destructive sampling, a-f: TOC calculation of 12 plots samples in 3 batches using TOC-V Analyzer.
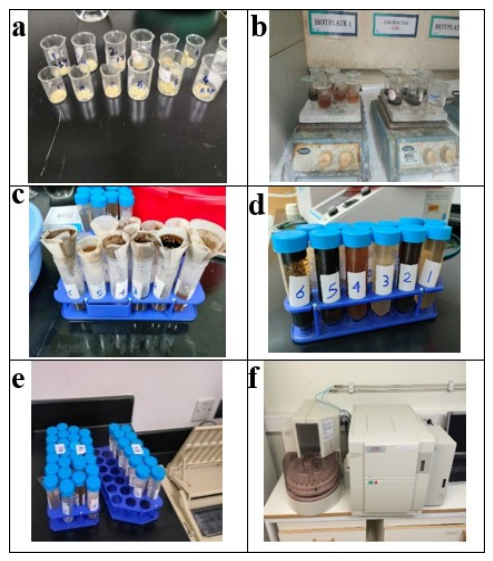
Figure 3.
Destructive sampling of Phragmites australis (Reed grass): targeted Plots number (position) verse fresh weight/plot (g, left y-axis), reed height (m, right y-axis) and number of reeds per plot (No, secondary axis).
Figure 3.
Destructive sampling of Phragmites australis (Reed grass): targeted Plots number (position) verse fresh weight/plot (g, left y-axis), reed height (m, right y-axis) and number of reeds per plot (No, secondary axis).
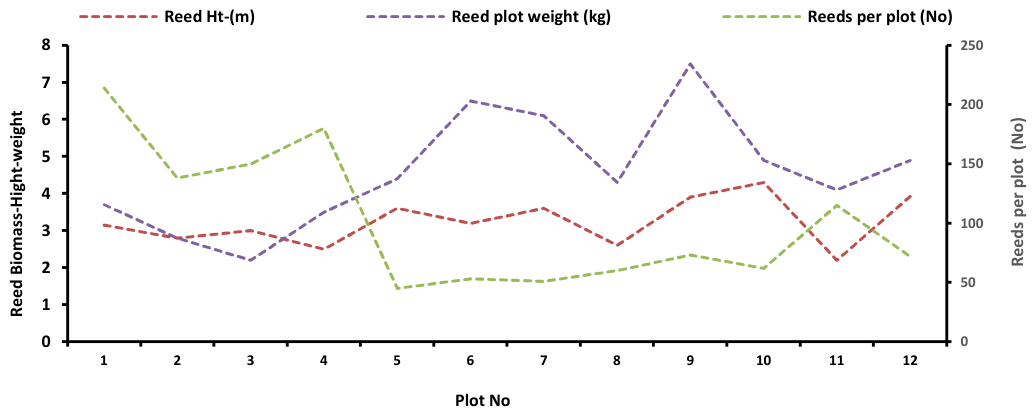
Figure 4.
Destructive sampling of Phragmites australis (Reed grass): targeted Plots number (position) verse Reed AGB (kg/m², left y-axis, dry-ratio approach), reed height (m) and Reed plot fresh weight/plot (kg, secondary axis).
Figure 4.
Destructive sampling of Phragmites australis (Reed grass): targeted Plots number (position) verse Reed AGB (kg/m², left y-axis, dry-ratio approach), reed height (m) and Reed plot fresh weight/plot (kg, secondary axis).
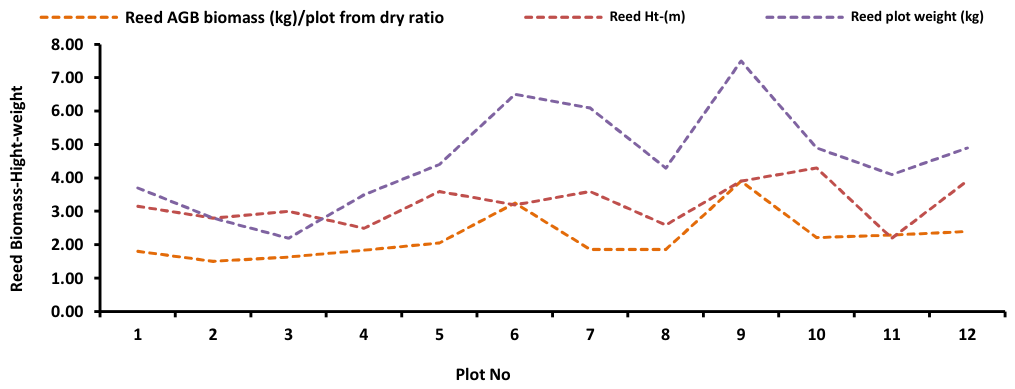
Figure 5.
Destructive sampling of Phragmites australis (Reed grass): targeted Plots number (position) verse Reed AGB (kg/m², left y-axis, TOC approach), reed height (m) and Reed plot fresh weight/plot (kg, secondary axis).
Figure 5.
Destructive sampling of Phragmites australis (Reed grass): targeted Plots number (position) verse Reed AGB (kg/m², left y-axis, TOC approach), reed height (m) and Reed plot fresh weight/plot (kg, secondary axis).
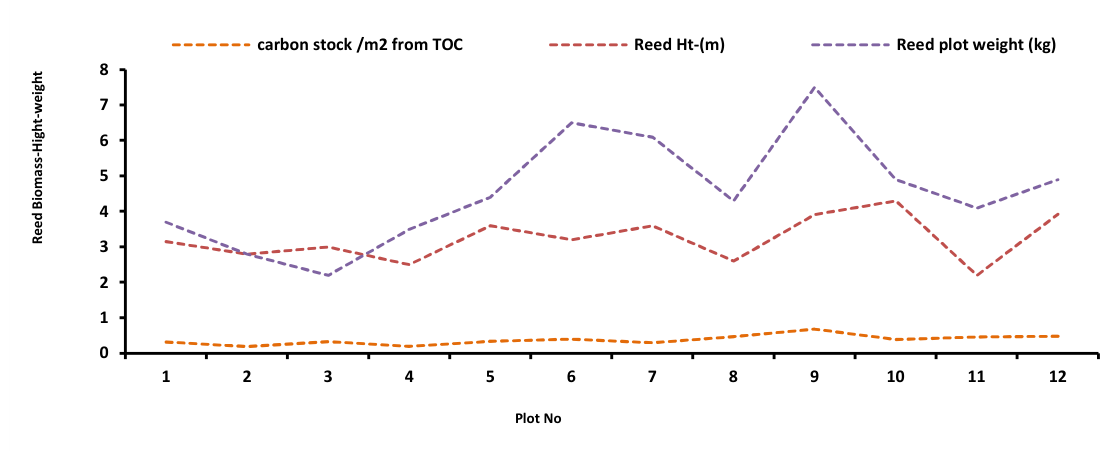
Figure 6.
Destructive sampling of Phragmites australis (Reed grass): Lab calculated dry weight over days (out of 12 plots) verse samples fresh-dry (moisture loss) wight (g).
Figure 6.
Destructive sampling of Phragmites australis (Reed grass): Lab calculated dry weight over days (out of 12 plots) verse samples fresh-dry (moisture loss) wight (g).
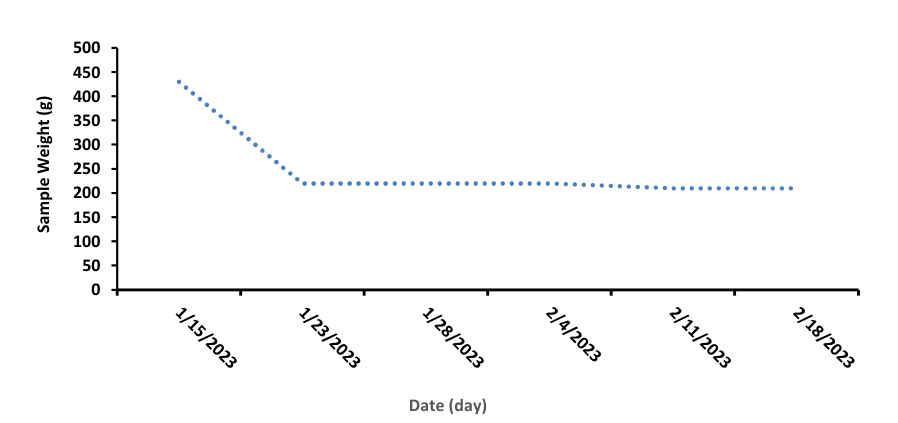
Figure 7.
Destructive sampling of Phragmites australis (Reed grass): Total organic carbon output of 12 plots using TOC-V Analyzer (No) verses three batches TOC in (%).
Figure 7.
Destructive sampling of Phragmites australis (Reed grass): Total organic carbon output of 12 plots using TOC-V Analyzer (No) verses three batches TOC in (%).
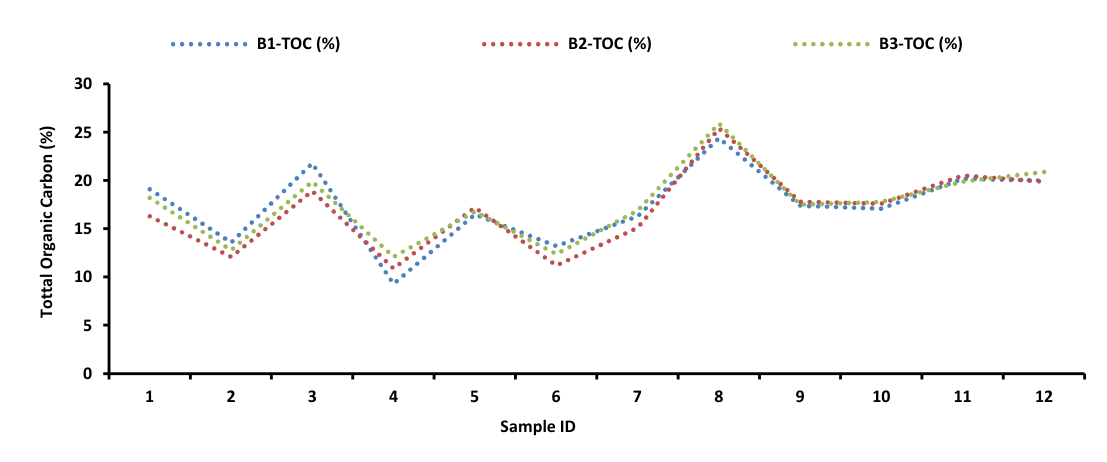
Figure 8.
Destructive sampling of Phragmites australis (Reed grass): Comparison of targeted plots (No) verses AGB carbon stock/m2 out of two-way approach.
Figure 8.
Destructive sampling of Phragmites australis (Reed grass): Comparison of targeted plots (No) verses AGB carbon stock/m2 out of two-way approach.
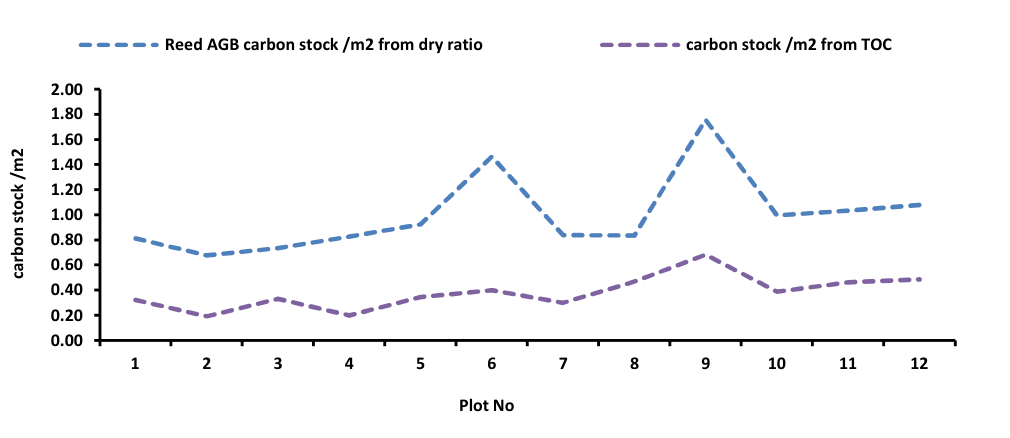
Figure 9.
Matrix plot Correlation of Phragmites australis (Reed grass) novel models of AGB verses plant measured variables.
Figure 9.
Matrix plot Correlation of Phragmites australis (Reed grass) novel models of AGB verses plant measured variables.
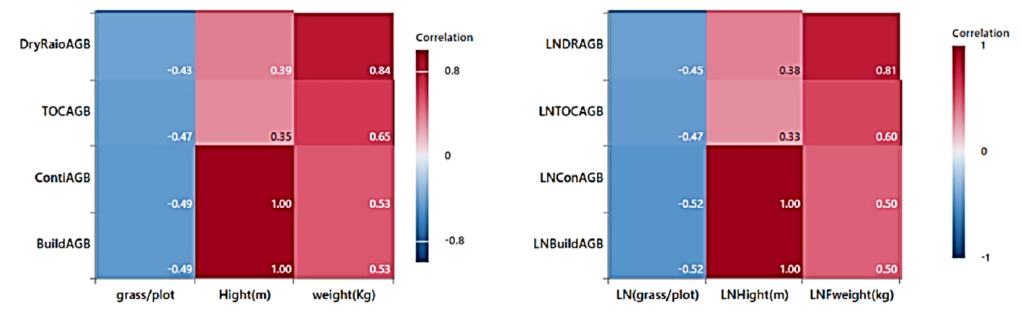
Figure 10.
Matrix plot Correlation of Phragmites australis (Reed grass) novel models of AGB verses plant measured variables in 2D.
Figure 10.
Matrix plot Correlation of Phragmites australis (Reed grass) novel models of AGB verses plant measured variables in 2D.
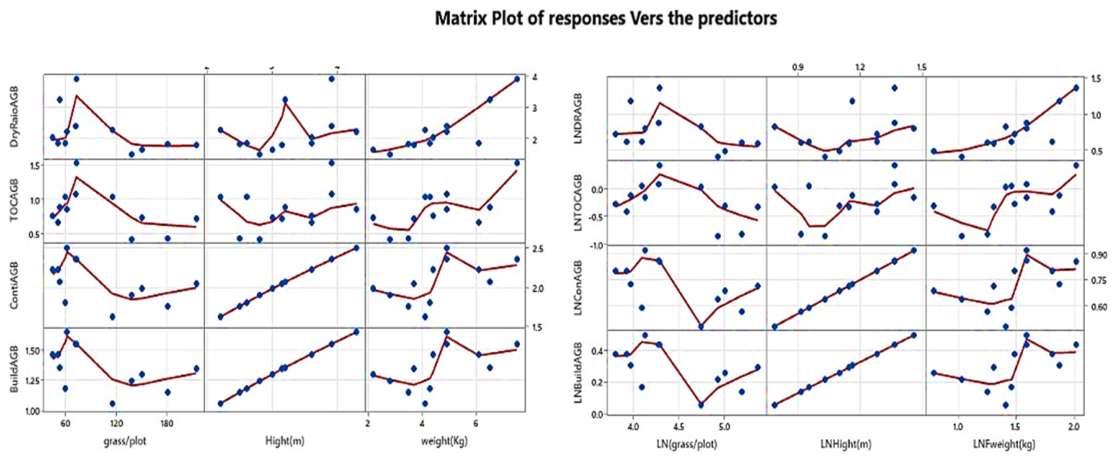
Figure 11.
Correlation of Phragmites australis (Reed grass) AGB verses plant measured plots of destructive sampling along fitted study equations and calculated biomass Approach.
Figure 11.
Correlation of Phragmites australis (Reed grass) AGB verses plant measured plots of destructive sampling along fitted study equations and calculated biomass Approach.
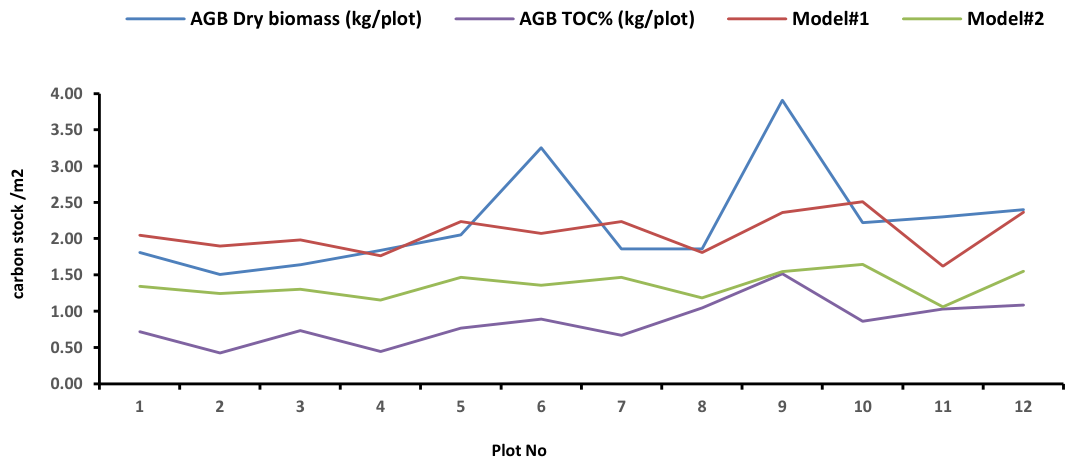
Figure 12.
Reed height plotted against destructively measured AGB (Table 2) and against the AGB values predicted by the two height-based allometric equations (Model#1, from Conti et al. [2019]; Model#2, this study’s recalibration of that equation). The near-perfect fit of both model-predicted series reflects their mathematical dependence on height rather than independent validation; see Discussion for the correlation between height and the destructively measured AGB values.
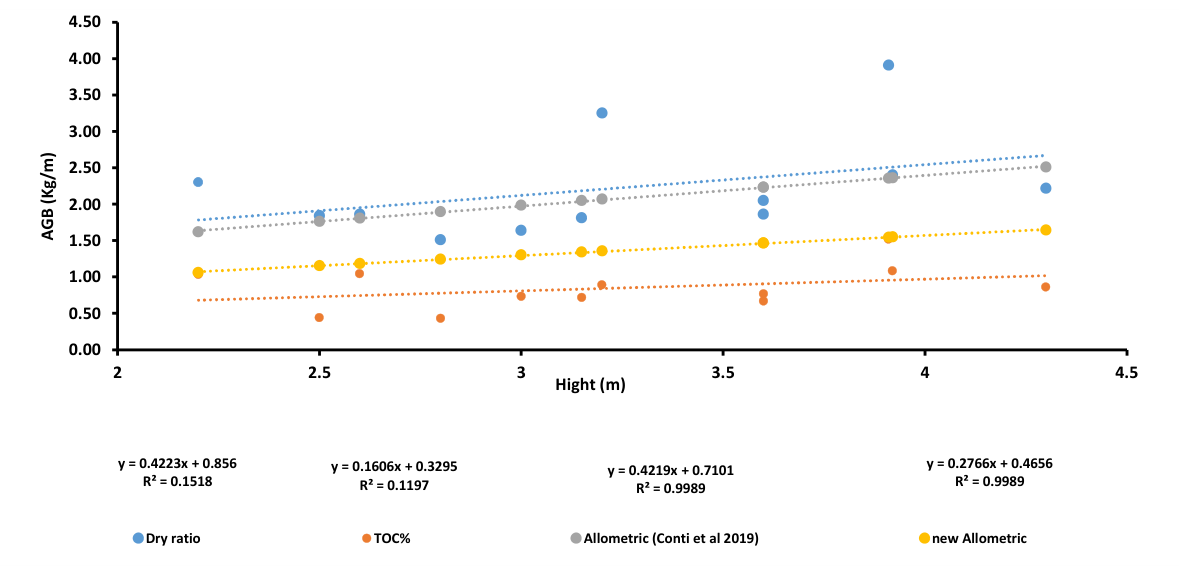
Figure 13.
The evaluation of correlated studies and measured AGB along destructive reeds verses the weight predictor.
Figure 13.
The evaluation of correlated studies and measured AGB along destructive reeds verses the weight predictor.
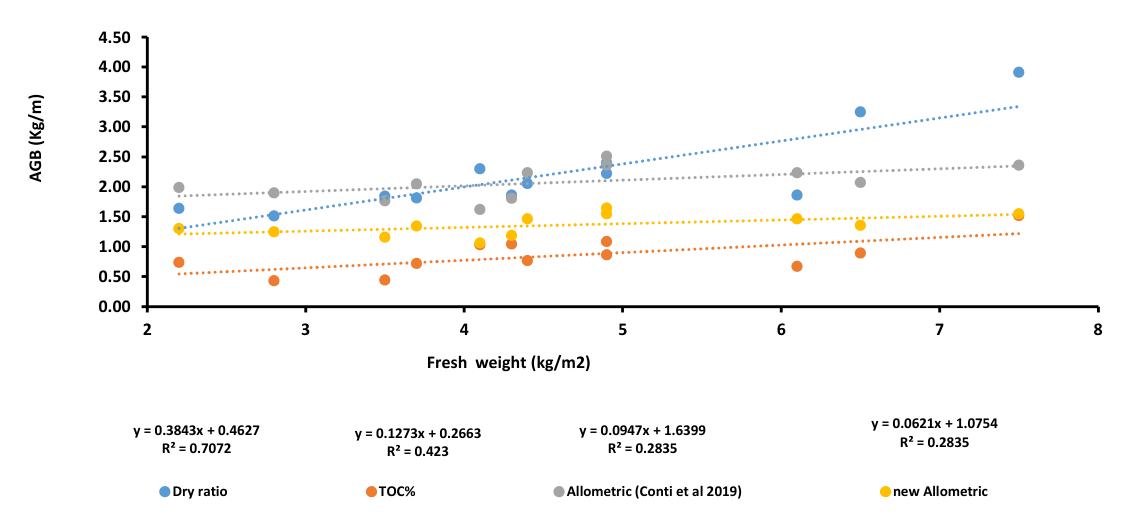
Figure 14.
The evaluation of correlated studies and measured AGB along destructive reeds verses the number of Reeds per plot predictor.
Figure 14.
The evaluation of correlated studies and measured AGB along destructive reeds verses the number of Reeds per plot predictor.
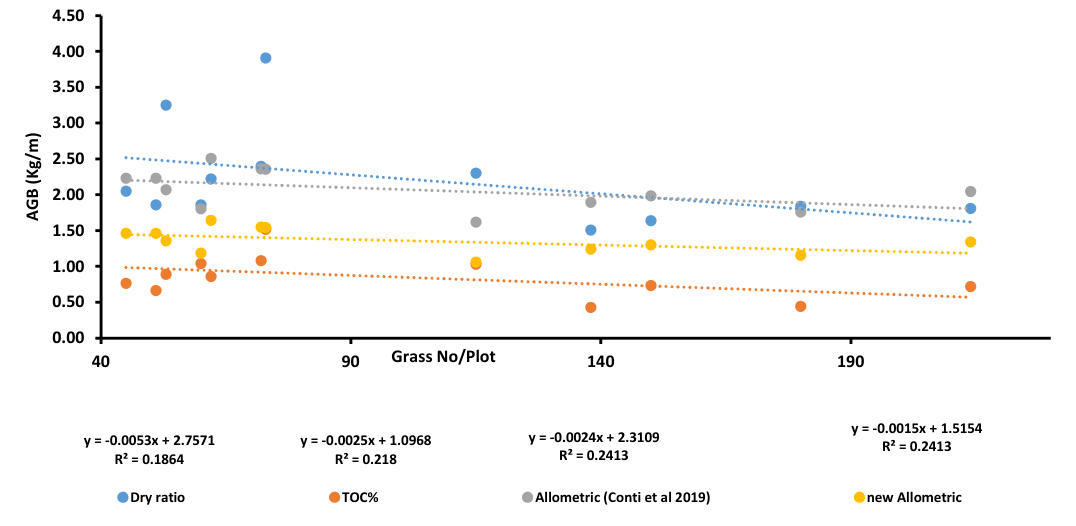
Figure 15.
Correlation of Phragmites australis (Reed grass) Novel models of AGB Log’s verses Log reeds measured height variable.
Figure 15.
Correlation of Phragmites australis (Reed grass) Novel models of AGB Log’s verses Log reeds measured height variable.
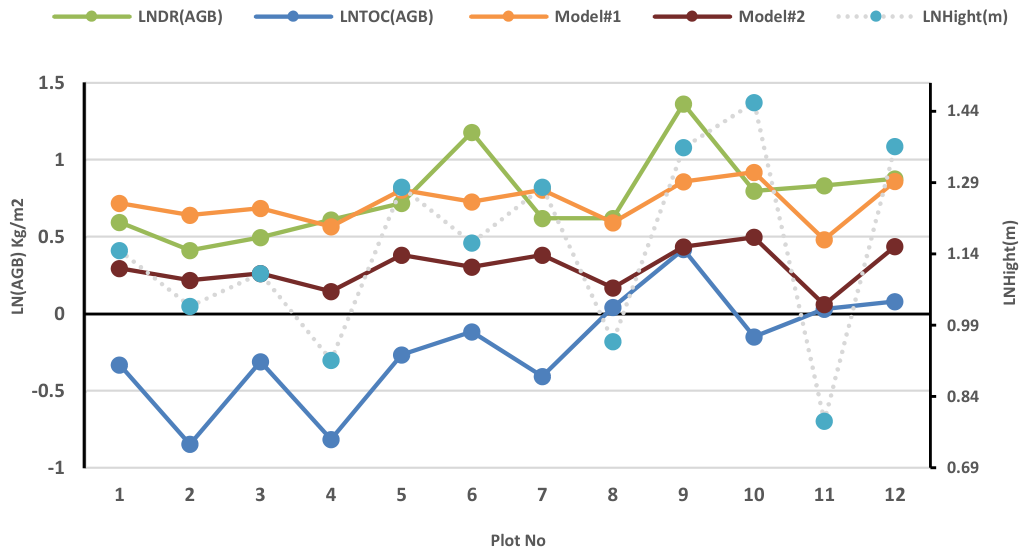
Figure 16.
Matrix plot Correlation of Phragmites australis (Reed grass) Novel models of AGB Log’s verses Log plant measured height variable.
Figure 16.
Matrix plot Correlation of Phragmites australis (Reed grass) Novel models of AGB Log’s verses Log plant measured height variable.
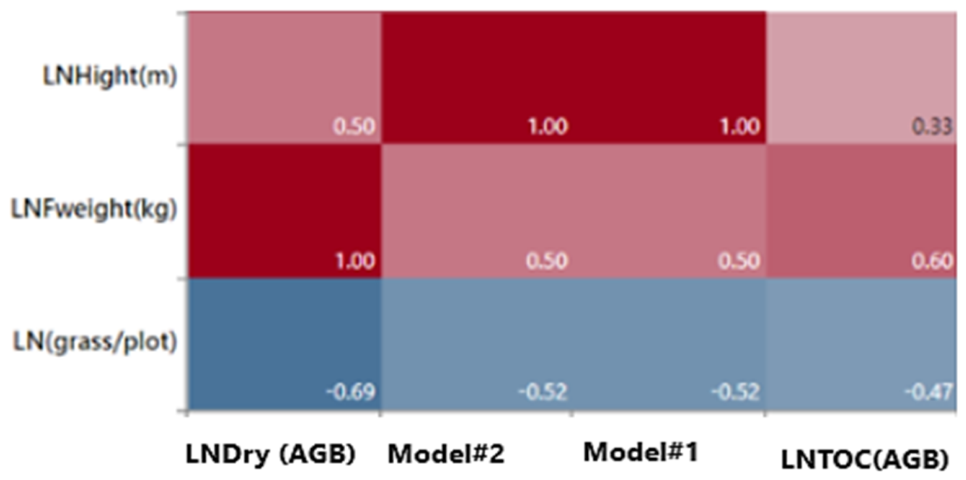
Figure 17.
Destructive (Obs) to Model-1 performance fitness chart.
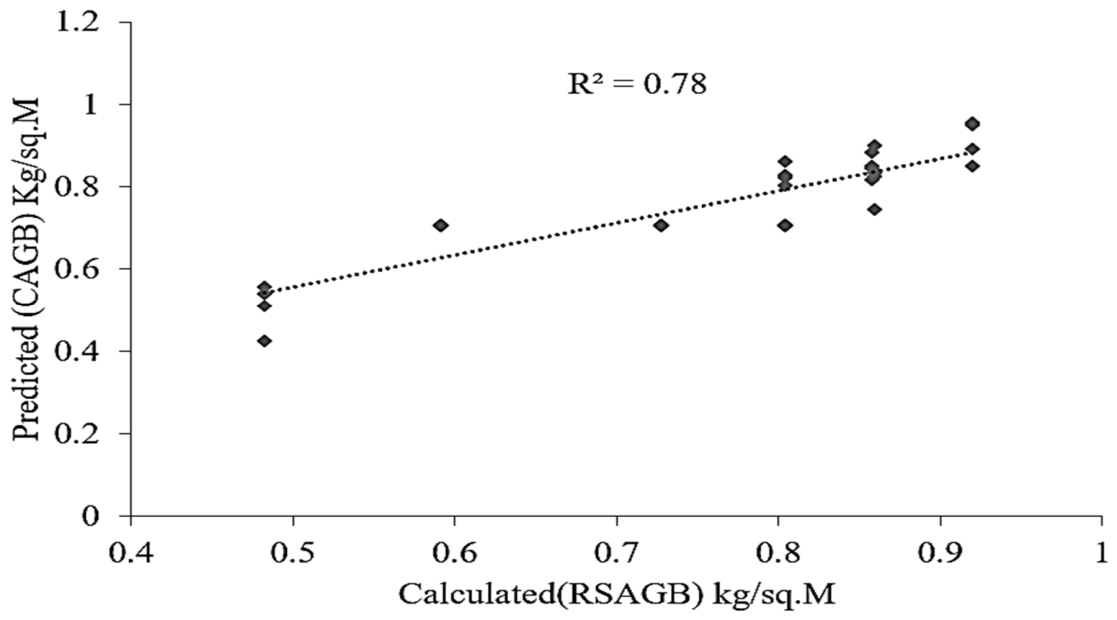
Figure 18.
RSAGB estimated for Reed plants using satellite imagery. (a) Overall imagery, (b) zoomed imagery.
Figure 18.
RSAGB estimated for Reed plants using satellite imagery. (a) Overall imagery, (b) zoomed imagery.
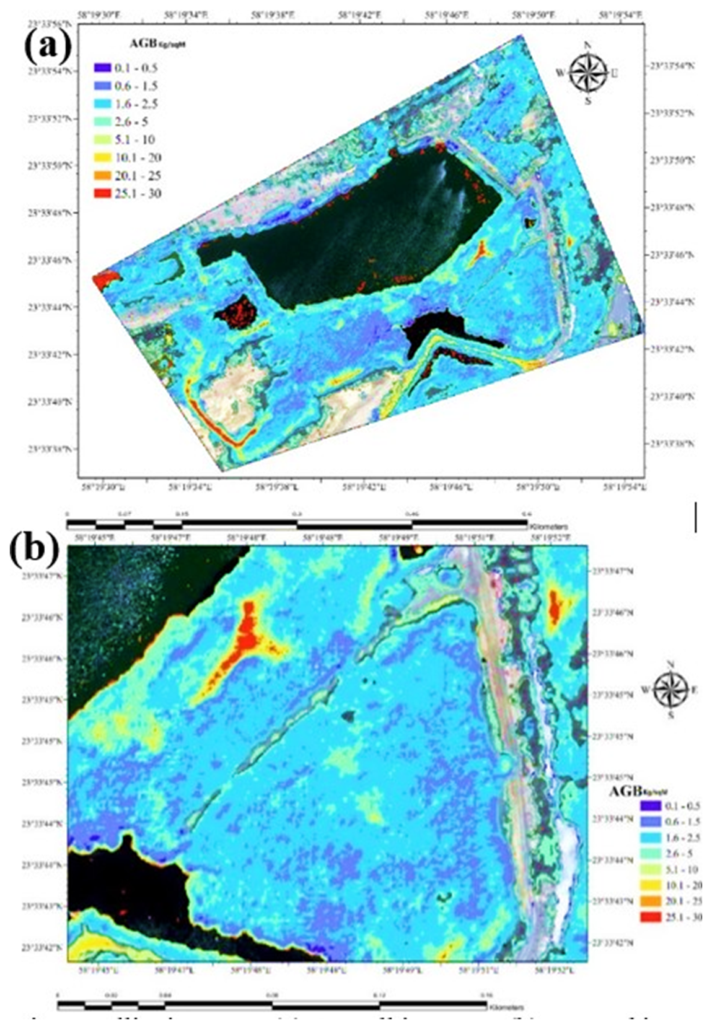
Figure 19.
RS-Carbon-Seq. estimated using satellite imagery for the Reed plants. (a) Overall imagery, (b) zoomed imager.
Figure 19.
RS-Carbon-Seq. estimated using satellite imagery for the Reed plants. (a) Overall imagery, (b) zoomed imager.
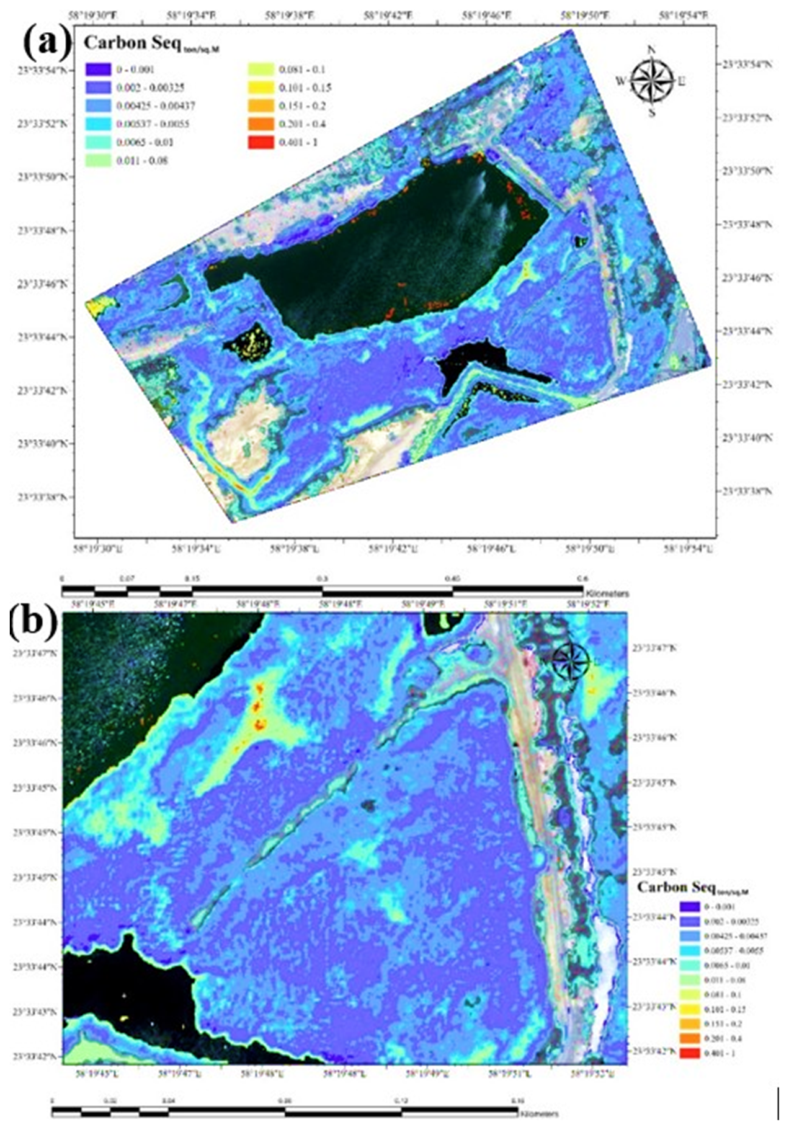
Figure 20.
Overall workflow of the study methodology, from field destructive sampling and laboratory analysis through allometric regression modelling and satellite-based remote sensing to the correlation of the two approaches.
Figure 20.
Overall workflow of the study methodology, from field destructive sampling and laboratory analysis through allometric regression modelling and satellite-based remote sensing to the correlation of the two approaches.
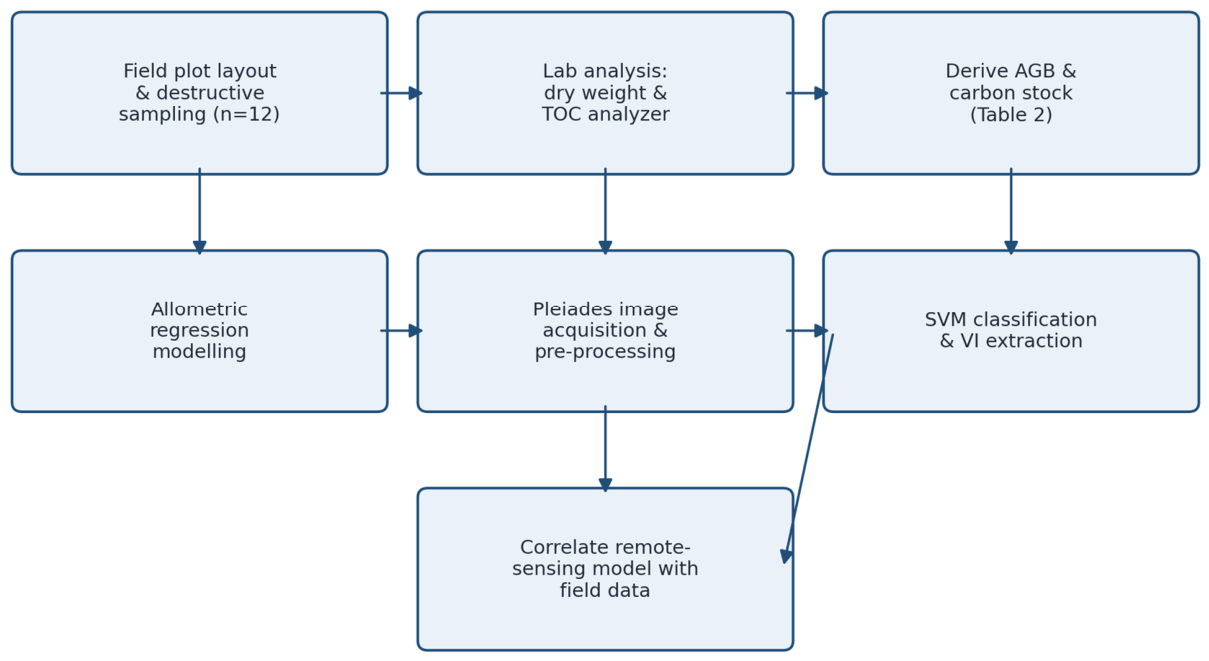
Figure 21.
Phragmites australis study area.
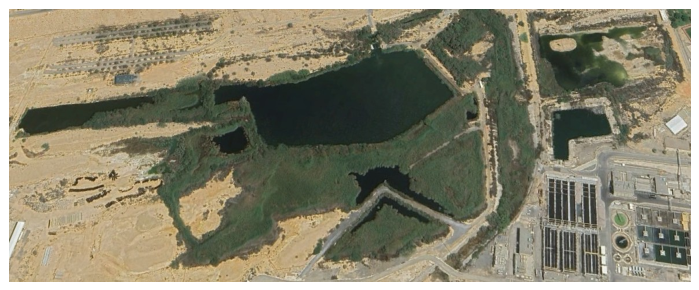
Figure 22.
The location site (red square) of Phragmites australis study area in Oman.
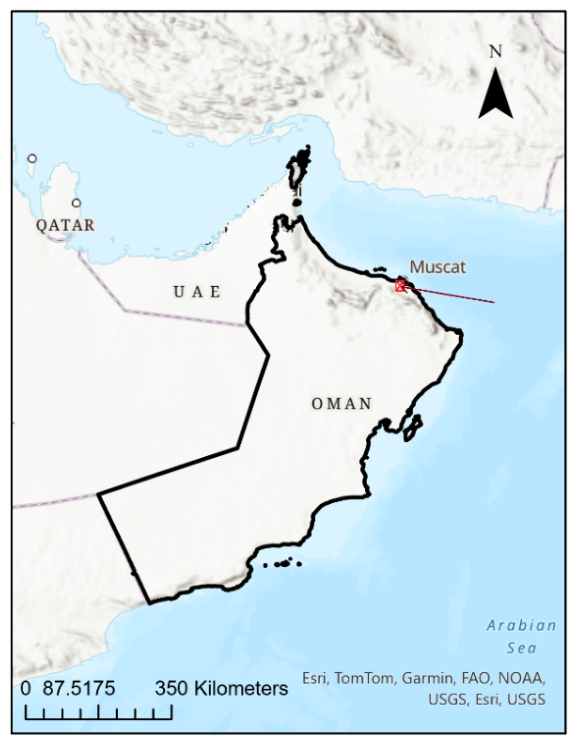
Figure 23.
Field measurements and operational procedures depicted.
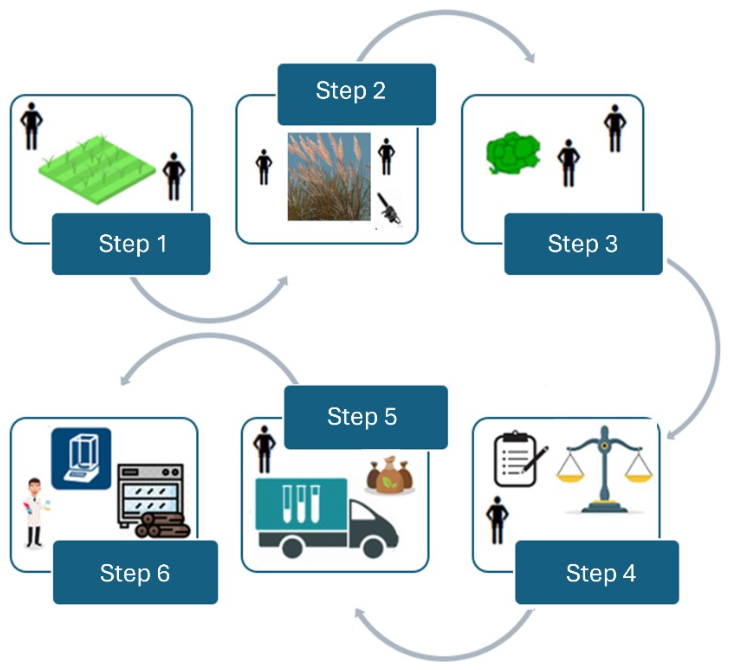
Figure 24.
Summary of the approach and analysis steps followed in this study.
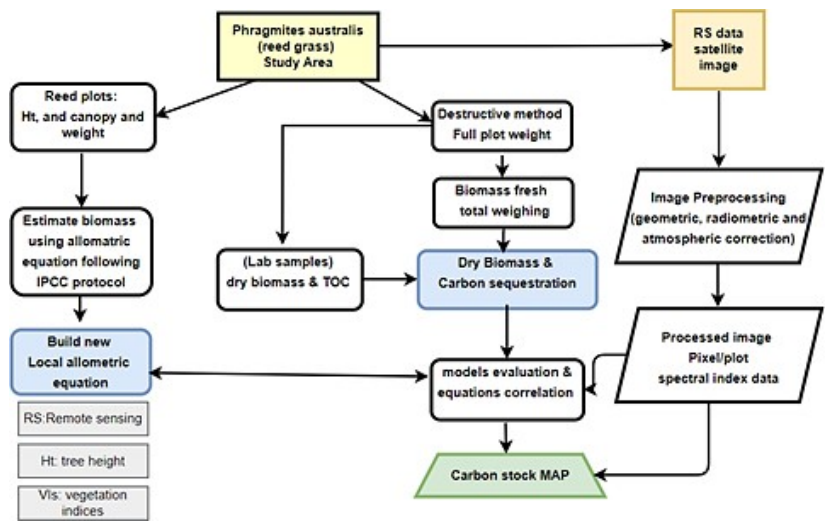

Table 1.
List of Actual destructive Phragmites australis (Reed grass) plots measurements results, Ht: reed high, Et: weight.
Table 1.
List of Actual destructive Phragmites australis (Reed grass) plots measurements results, Ht: reed high, Et: weight.
| Plot No | Plot size (m) |
Reeds Hight (m) |
Reeds per plot (No) |
Reeds Plot fresh weight (kg) |
Sample dry weight (g) |
| 1 | 1 * 1 | 3.15 | 214 | 3.7 | 430 |
| 2 | 1 * 1 | 2.8 | 138 | 2.8 | 390 |
| 3 | 1 * 1 | 3 | 150 | 2.2 | 390 |
| 4 | 1 * 1 | 2.5 | 180 | 3.5 | 380 |
| 5 | 1 * 1 | 3.6 | 45 | 4.4 | 450 |
| 6 | 1 * 1 | 3.2 | 53 | 6.5 | 340 |
| 7 | 1 * 1 | 3.6 | 51 | 6.1 | 360 |
| 8 | 1 * 1 | 2.6 | 60 | 4.3 | 370 |
| 9 | 1 * 1 | 3.91 | 73 | 7.5 | 480 |
| 10 | 1 * 1 | 4.3 | 62 | 4.9 | 420 |
| 11 | 1 * 1 | 2.2 | 115 | 4.1 | 500 |
| 12 | 1 * 1 | 3.92 | 72 | 4.9 | 490 |
Table 2.
List of Actual destructive Phragmites australis (Reed grass) plots measurements using two-way approach, Ht: reed height, Et: weight.
Table 2.
List of Actual destructive Phragmites australis (Reed grass) plots measurements using two-way approach, Ht: reed height, Et: weight.
| Dry weight Ratio Approach | TOC Approach | ||||||
| Plot No | Reed wet-dry ratio | Reed AGB kg/m2 from dry ratio | Reed Carbon stock kg/m2 from dry ratio | TOC % | carbon stock kg/m2 from TOC Analyzer | ||
| 1 | 0.488 | 1.81 | 0.90 | 17.9 | 0.6623 | ||
| 2 | 0.538 | 1.51 | 0.75 | 12.8 | 0.3584 | ||
| 3 | 0.744 | 1.64 | 0.82 | 20.2 | 0.4444 | ||
| 4 | 0.526 | 1.84 | 0.92 | 10.8 | 0.378 | ||
| 5 | 0.467 | 2.05 | 1.03 | 16.8 | 0.7392 | ||
| 6 | 0.500 | 3.25 | 1.63 | 12.3 | 0.7995 | ||
| 7 | 0.306 | 1.86 | 0.93 | 16.1 | 0.9821 | ||
| 8 | 0.432 | 1.86 | 0.93 | 25.2 | 1.0836 | ||
| 9 | 0.521 | 3.91 | 1.95 | 17.5 | 1.3125 | ||
| 10 | 0.452 | 2.22 | 1.11 | 17.5 | 0.8575 | ||
| 11 | 0.560 | 2.30 | 1.15 | 20.2 | 0.8282 | ||
| 12 | 0.490 | 2.40 | 1.20 | 20.3 | 0.9947 | ||
| Average Carbon stock: | 1.11 | 0.7867 | |||||
Table 3.
List of Actual destructive Phragmites australis (Reed grass) plots measurements using two-way approach, Ht: reed height, Et: weight.
Table 3.
List of Actual destructive Phragmites australis (Reed grass) plots measurements using two-way approach, Ht: reed height, Et: weight.
| AGB | comments | Method/Location | Reference |
| 2.22 kg/m2 AGB | 1.11 kg/m2 C | Dry/fresh ratio approach | This Study |
| 0.79 kg/m2 C* | TOC approach | ||
| 1.853 kg/m2 | 3.3-1.46 (80% BGB) | dry samples | [43] |
| 0.642 kg/m2 | 3.0–35.6 kg/m2 in | Pristine Salt Marsh | |
| 1.04 kg/m2 | 8.6–24.0 kg/m2 in | Impacted Salt Marsh | [44] |
| 0.31–52.90 Mg/ha (mean: 0.733 kg/m2) |
[42,45] | ||
| 30.4(MT ha-1 Year-1) 3.04 kg/m2 | Egypt | [46] | |
| 13.6 (MT ha-1 Year-1) 1.36 kg/m2 | Iraq | [47] | |
| 16.8 (MT ha-1 Year-1) 1.68 kg/m2 | Minnesota | [48] | |
| 9.9-25.1 (MT ha-1 Year-1) 0.99-2.51 kg/m2 | Sweden | [49] |
*0.50 a carbon factor used. Note: values in this table are reported in the original units used by each cited source. Conversion factors applied for comparison in the text: 1 Mg/ha = 0.1 kg/m²; 1 MT ha⁻¹ year⁻¹ (dry biomass, oven-dry basis) = 0.1 kg/m² year⁻¹.
Table 4.
The list of Phragmites australis (Reed grass) AGB logarithms driven regression models using the measured plants plots (n=12).
Table 4.
The list of Phragmites australis (Reed grass) AGB logarithms driven regression models using the measured plants plots (n=12).
|
Plots (12) Model#1 Stepwise |
Regression Equation Model AGB=-0.03139 + 0.6520 LN Hight(m) |
Variables H |
R-sq (pred) 100.0% |
P-Value Fit |
|
| Model#2 Stepwise |
AGB=-0.4534 + 0.6520 LN Hight (m) | H | 100.0% | Fit | |
| LN Dry | AGB=-0.90 + 0.030 LN Hight(m) + 0.756 LNF weight(kg) | H&W | 24.07% | 0.022:0.9280.10&0.4 | |
| Regression (AGB) Stepwise LN TOC |
+ 0.114 LN (grass/plot) -0.183+ 0.642 LNF weight(kg) AGB=-0.78 + 0.038 LN Hight(m) + 0.547 LNF weight(kg) |
W H&W |
40.21% 0.00% |
0.001:0.001 0.275:0.951,0.226, |
|
| Regression (AGB) Stepwise |
- 0.064 LN (grass/plot) -1.141 + 0.626 LNF weight(kg) |
RN & W |
0.00% | 0.039:0.039 | |
Table 5.
The list of novel Models of three targeted species on the estimations of Above ground biomass using statistical correlation regression modelling analysis.
Table 5.
The list of novel Models of three targeted species on the estimations of Above ground biomass using statistical correlation regression modelling analysis.
| species | Model (Ln (AGB)) | Variable | Model No |
| Phragmites australis | AGB=-0.03139+ 0.6520 LNHight(m) AGB=-0.4534 + 0.6520 LNHight(m) |
H H |
1 2 |
Table 6.
Models performance fitness to the destructive sampling (Dry biomass and TOC methods).
| Models’ fitness to Destructive Dry Biomass | R2 | MAE | RMSE | RE | MAPE |
| Model-1 | 0.156 | 0.193 | 0.248 | -3.8% | 25.2% |
| Model-2 | 0.152 | 0.461 | 0.522 | - 46.1% | 58.5% |
| TOC | |||||
| Model-1 | 0.024 | 0.478 | 0.508 | 40.2% | 463.4% |
| Model-2 | 0.026 | 0.217 | 0.313 | -2.1% | 124.7% |
Table 7.
RS verses predicted Models fitness performance.
| Models’ fitness | R2 | MAE | RMSE | RE | MAPE |
| Model-1 | 0.781 | 0.054 | 0.066 | 0.20% | 7.90% |
| Model-2 | 0.783 | 0.053 | 0.065 | 0.20% | 27.80% |
Table 8.
List of some vegetation indices extracted and tested in the study.
| Vegetation Spectral Indices | Formula Definition | References |
| Red (R), Green (G), Blue (B) |
raw value of each band rn=R/(R+G+B); | / |
| Nomalized Red (rn), Green (gn), Blue (bn) |
rn=R/(R+G+B); gn=G/(R+G+B); bn=B/(R+G+B) | / |
| *Green, red ratio index (GRRI) |
GRRI=G/R | / |
| *Green blue ratio index |
GBRI=G/B | / |
| *Red, blue ratio index (RBRI) |
RBRI=R/B | / |
| *Color intensity index (CII) |
INT = (R+G+B)/3 | [50] |
| Green leaf index | GLI = (2×G−R−B)/(2×G+R+B) | [51] |
|
*Visible atmospherically resistance index (VARI) |
VARI = (G−R)/(G+R−B) |
[52] |
| Vegetative index | VEG=G/(Ra×B(1−a)), a=0.667 | [53] |
|
* Normalized difference red edge (NDRE) |
NIR-RE/NIR+RE |
[54] |
| * Normalized difference vegetation index (NDVI) |
NIR-R/NIR+R | [55] |
| * Simple ratio vegetation index (SRVI) |
NIR/R | [56] |
| * Canopy chlorophyll content index (CCCI) |
NDRE/NDVI | [54] |
| SAVIcam (noise adjusted vegetation index) | (1.5N)(B-R) / (B+R+0.5N) | [57] |
|
*Transformed Soil Adjusted Vegetation Index |
(s *(NIR - s * Red - a)) / (a * NIR + Red - a * s + X * (1 + s2)) |
[58] |
Note: N = 255. while R, G, and B are mean of digital number (DN) of these respective bands.RE1 RED edge band 1 – *The tested index with good respond.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (http://creativecommons.org/licenses/by/4.0/).
Copyright: This open access article is published under a Creative Commons CC BY 4.0 license, which permit the free download, distribution, and reuse, provided that the author and preprint are cited in any reuse.